Understanding Symbiotic Relationships in the Field
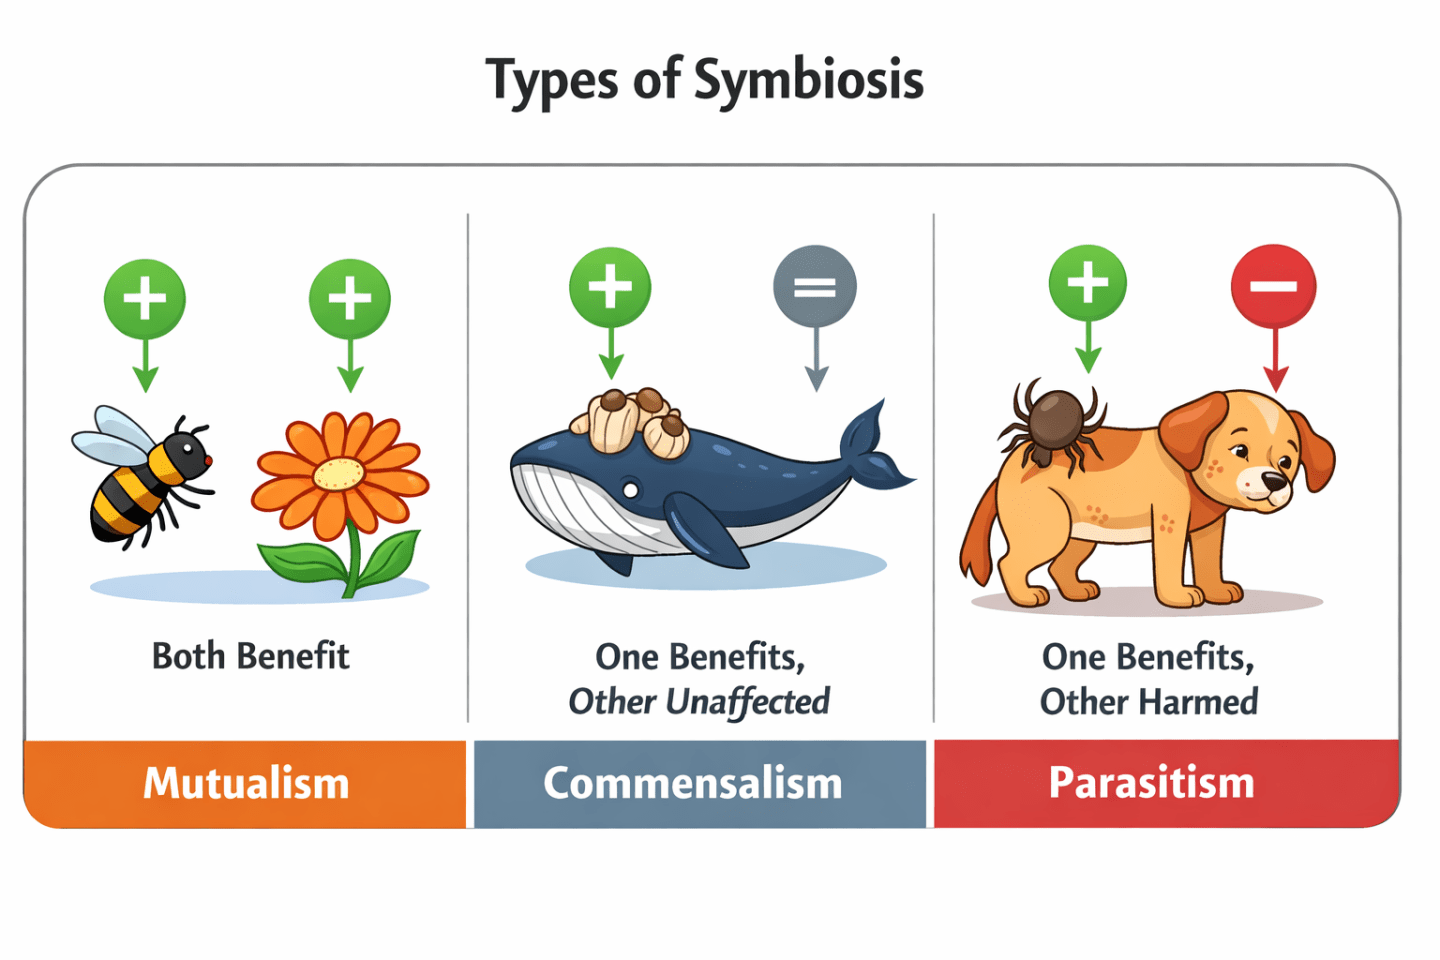
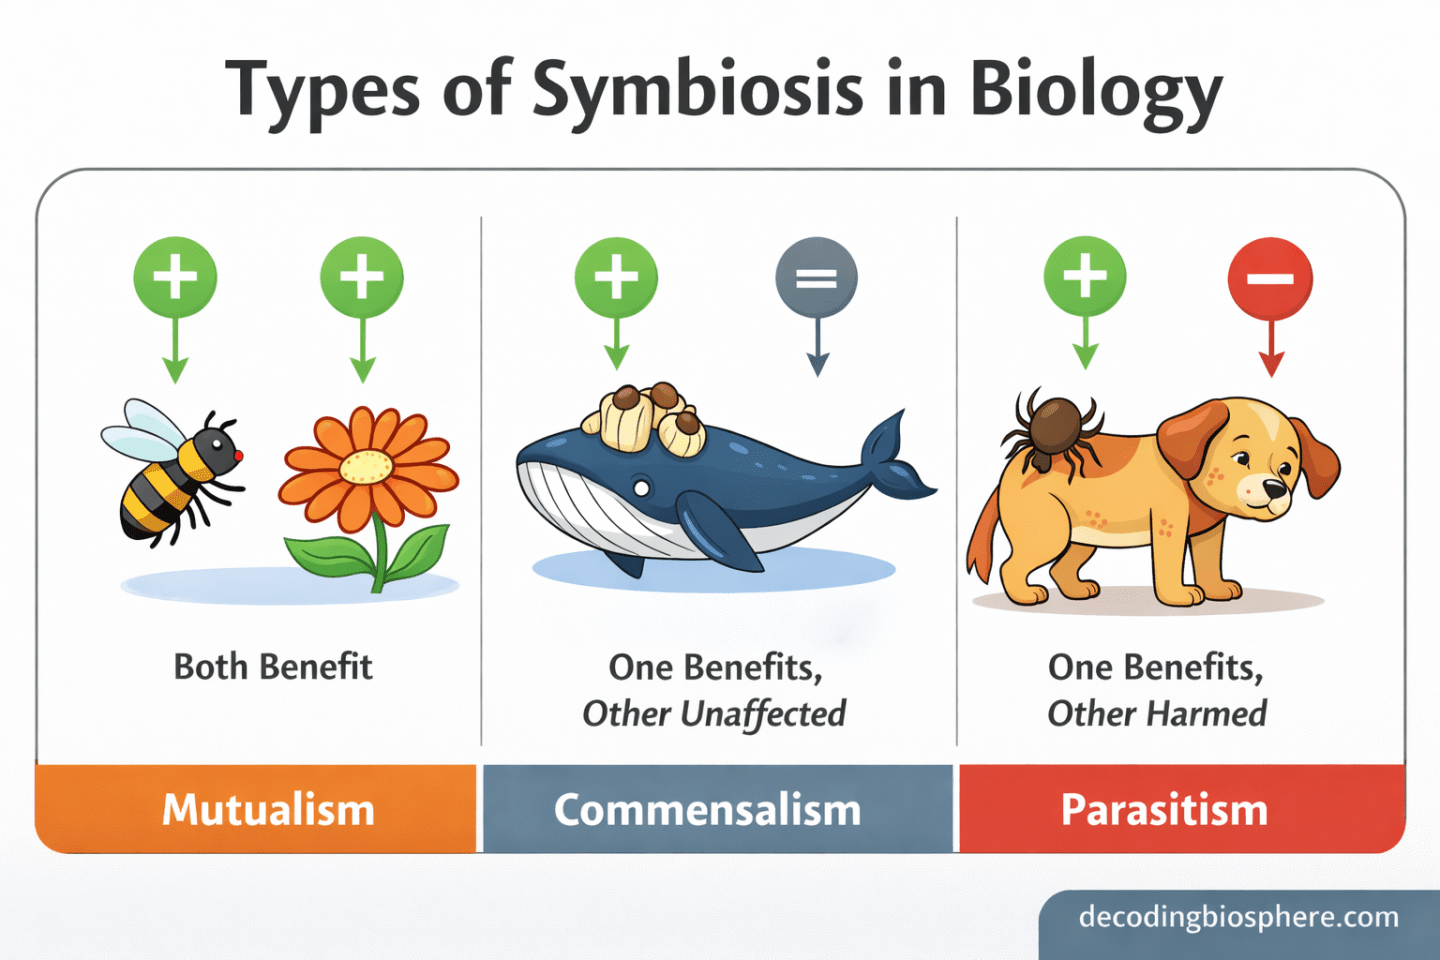
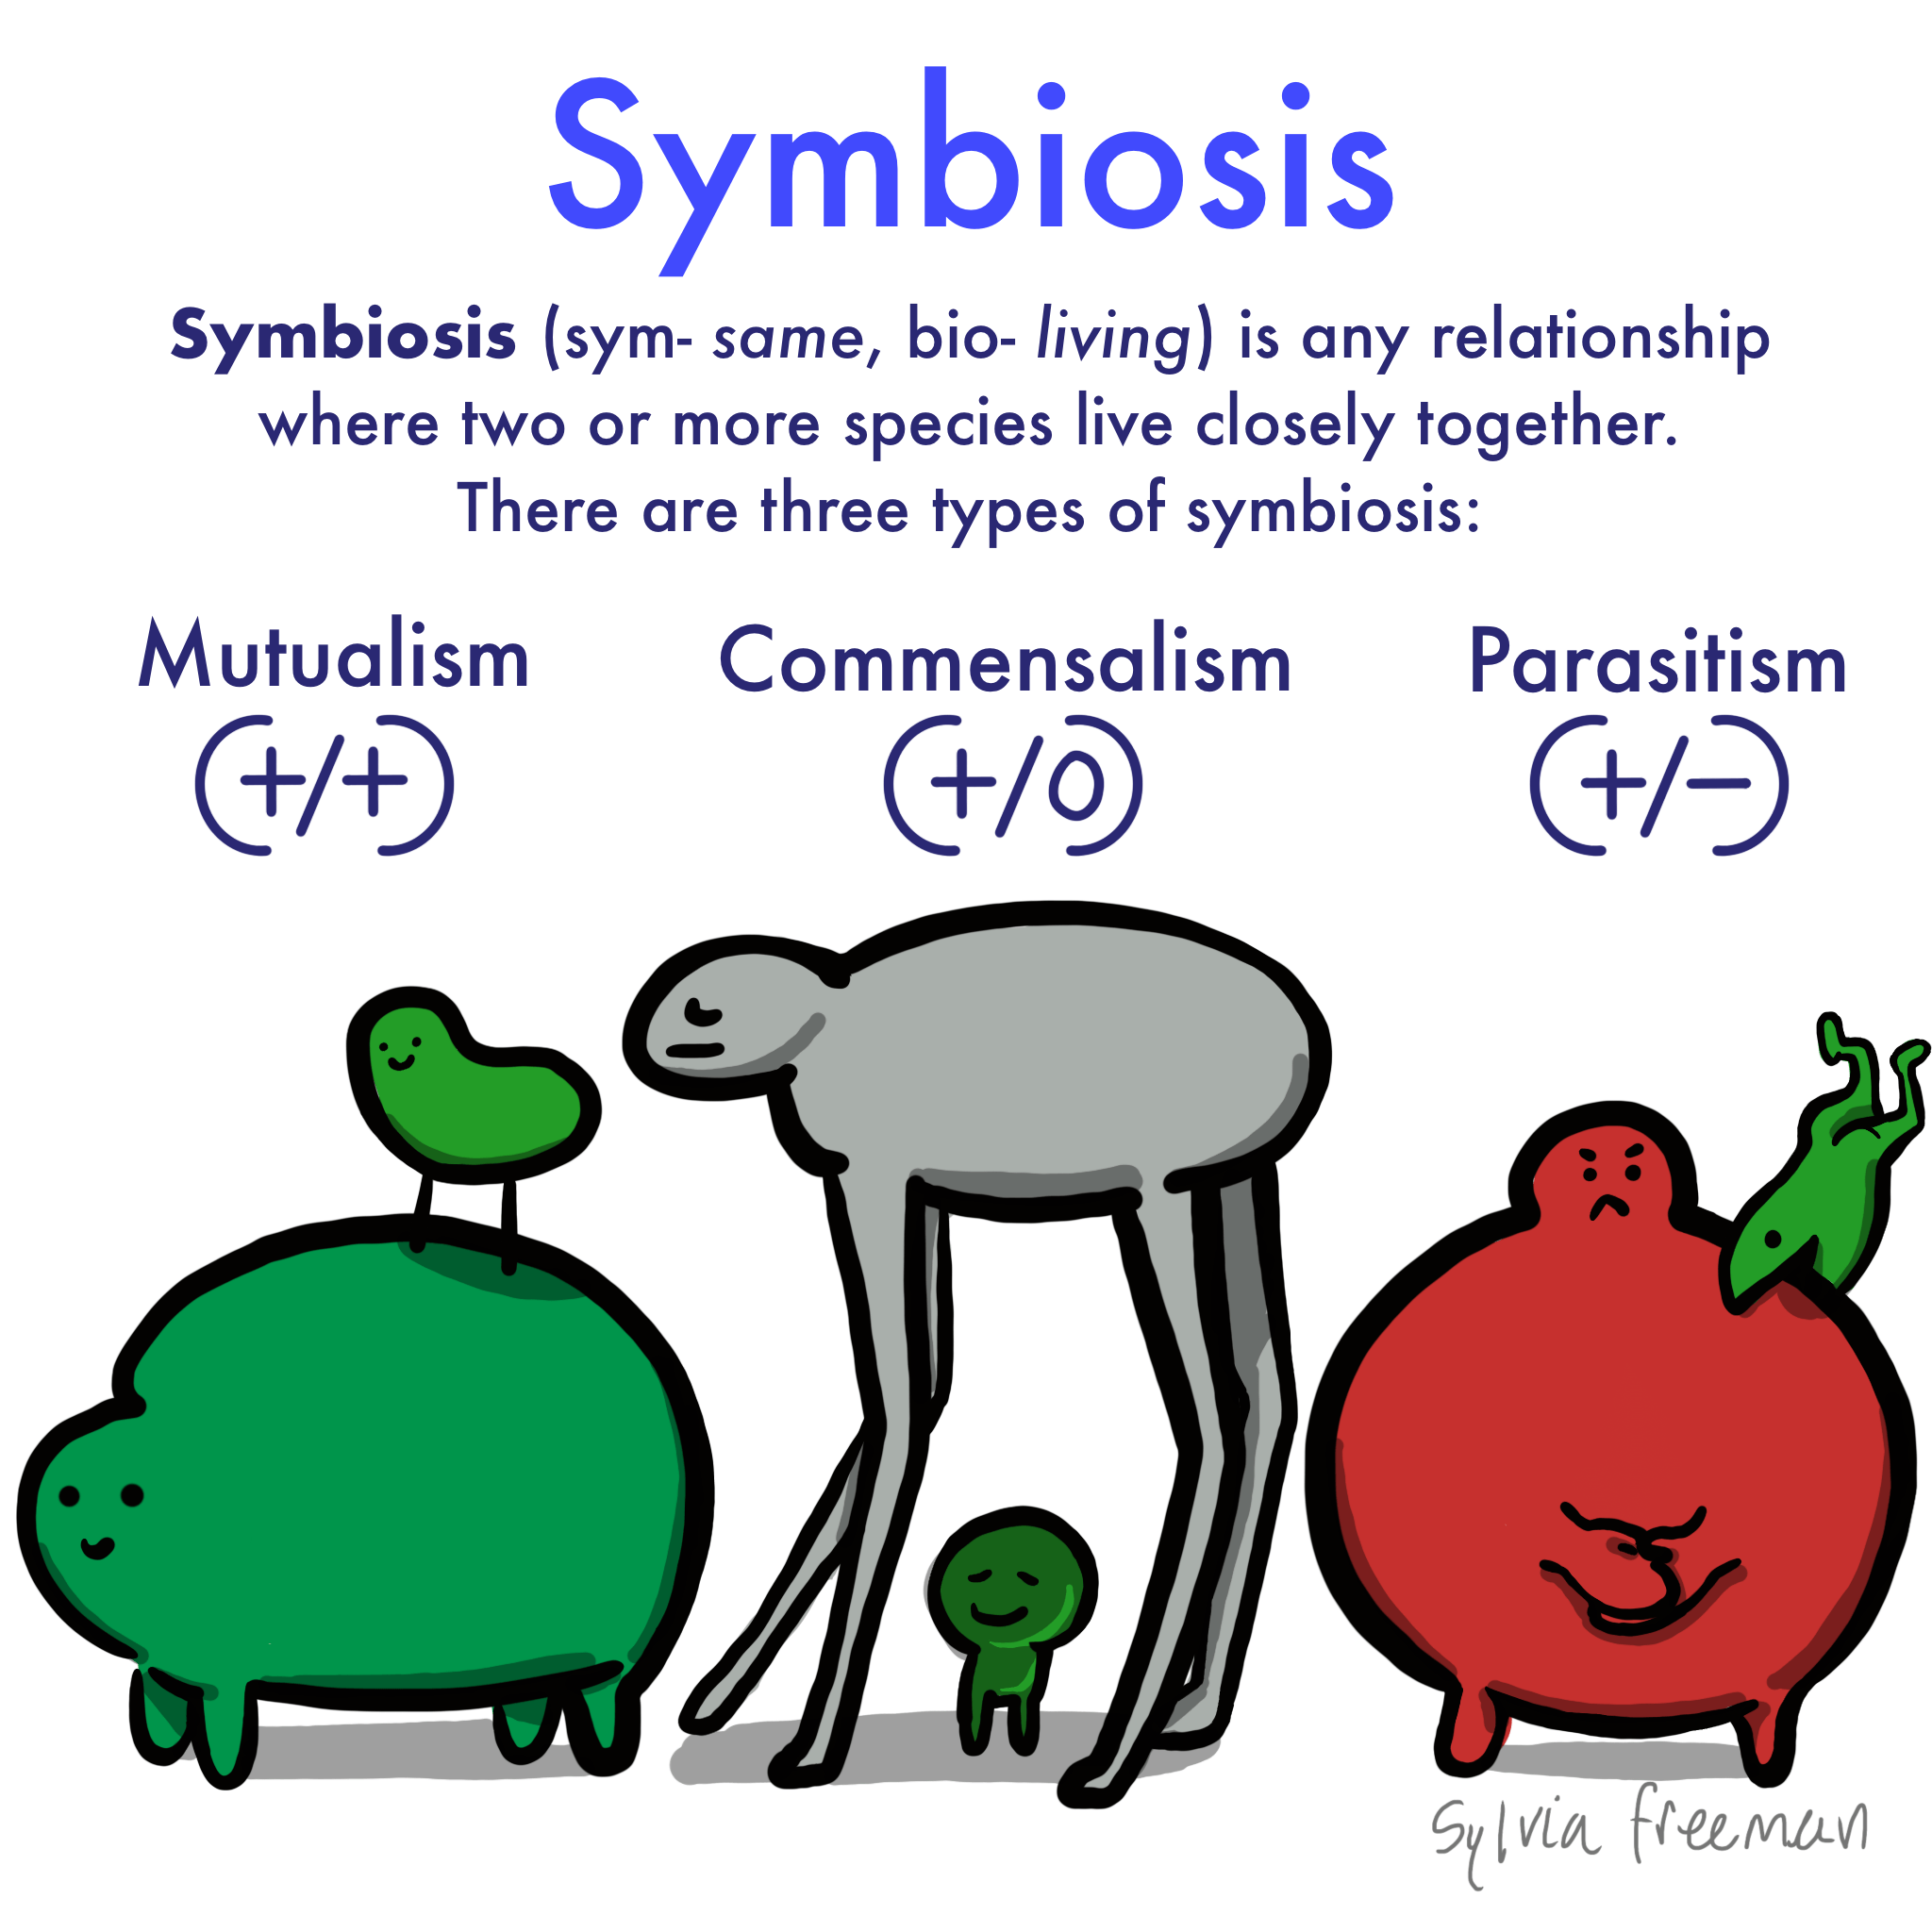
I ran into a real headache with this back when I was working with a coral reef monitoring project in the Philippines. We were trying to sequence the microbiome of certain symbiotic corals, and the protocols we used for free-living bacteria completely fell apart. The symbionts were too tightly bound to the host tissue, and our standard lysis buffers just couldn't separate them cleanly. What ended up working was a physical disruption step followed by a density gradient centrifugation, and even then, the success rate was maybe sixty percent per sample. That's the thing nobody tells you about studying symbiosis — the methods you use for regular microbial work almost never apply directly. Most textbooks present this as a simple three-way split, but the reality is messier. Mutualism is where both organisms benefit from the relationship. Commensalism describes a situation where one benefits and the other is neither helped nor harmed. Parasitism is the obvious one — one benefits at the expense of the other. That framework has been around since the late nineteenth century when Anton de Bary first coined the term, and it's still what you'll find in introductory courses. Here's where it gets less straightforward. The classification depends entirely on the balance of costs and benefits, and those shift constantly depending on environmental conditions. A relationship that looks mutualistic under one set of conditions can become parasitic under stress. I've seen lichen-forming fungi that switch from mutualistic to parasitic behavior when nutrient availability changes. The host-algal partnership breaks down, and the fungus starts digesting the algal cells instead of exchanging nutrients with them. This isn't a rare edge case. It happens frequently enough that anyone doing field work in symbiosis needs to account for it.
Practical Approaches to Studying Symbiotic Systems
If you're starting a project in this area, the first thing you need to figure out is whether the organisms you're looking at are facultatively or obligately symbiotic. Facultative symbionts can survive independently. Obligate symbionts cannot. This distinction determines everything about your experimental design. With obligate relationships, you're working with something that will die if you handle it wrong. Standard culturing techniques won't work because the symbiont often requires signals from the host to survive outside the host environment. For obligate symbionts, I recommend starting with molecular methods rather than culture-based approaches. Metagenomic sequencing combined with fluorescence in situ hybridization gives you a much clearer picture of what's actually happening inside the host. The culture-based approach has a huge blind spot — most symbiotic bacteria are unculturable using standard laboratory media. You could spend months trying to grow something that simply won't grow outside its host context. That's not a problem with your technique. It's a fundamental property of the relationship. When I was dealing with that nematode project I mentioned earlier, the workaround involved switching to a gentle homogenization method instead of bead-beating, which was destroying the symbiont cell walls, and then immediately running the lysate through a sucrose density gradient. The gradient separated the host cellular debris from the symbionts based on buoyant density. It took about forty-five minutes per sample instead of the ten minutes that bead-beating would have taken, but the recovery rate was significantly better. That's a real tradeoff you have to make consciously.
Common Pitfalls and Counter-Intuitive Observations
Beginners in this area tend to treat symbiosis as a fixed category. It's not. The same pair of organisms can exhibit different types of symbiotic interaction at different life stages or under different environmental pressures. Aphids and Buchnera bacteria are the classic example of obligate mutualism. The aphid provides a protected environment and nutrients. The bacterium provides essential amino acids the aphid can't get from its plant diet. But under certain temperature conditions, the relationship deteriorates. The bacteria start consuming more resources than they provide, and the aphid's fitness drops. You wouldn't classify that as mutualism if you observed it under heat stress. Another thing people miss is that commensalism is probably the hardest type to prove definitively. Just because you don't detect a cost or benefit doesn't mean one doesn't exist. Modern molecular techniques are sensitive enough to pick up effects that older methods would have completely missed. When I reviewed some older literature claiming commensal relationships, reanalysis with current techniques often revealed subtle parasitic or mutualistic effects that had gone undetected. The conclusion shifts from commensalism to something else once you have better tools. The third type, parasitism, has an interesting overlap with mutualism that isn't always acknowledged. Many parasites manipulate their host's behavior in ways that seem mutually beneficial from the host's limited perspective. Some parasitic wasps inject viruses along with their eggs that suppress the host's immune system. The host survives longer than it normally would after parasitization, which benefits the developing wasp larva. Without the viral suppression, the host would die too quickly. The line between parasite and mutualist blurs in situations like this.
Get the Full Details
When Standard Methods Break Down
There are scenarios where symbiosis research hits a wall. Host-associated symbionts with extremely reduced genomes — think of organisms like Carsonella ruddii, which has a genome smaller than some viruses — are nearly impossible to study with standard metagenomic approaches. The genome is so reduced that reference databases often don't have close matches. Assembly becomes a nightmare because the symbiont DNA is a tiny fraction of the total host sample, and the sequencing depth required to get coverage becomes prohibitively expensive. If you're working with systems like this, consider single-cell genomics as an alternative. It bypasses the assembly problem by reading individual cells rather than trying to piece together a mixed population. The downside is that it's expensive and low-throughput. You're looking at maybe twenty to fifty cells per run on a typical setup, which may not be representative of the full symbiont population. For many applications, that's acceptable. For others, it's a serious limitation. The three types of symbiosis framework is a useful starting point, but it shouldn't be treated as an endpoint. The relationships are dynamic, context-dependent, and often asymmetric across time scales. The organisms themselves don't care about your classification system. They're just trying to survive and reproduce, and sometimes that means partnering with another organism in ways that don't fit neatly into any box.