The Difference Between Active And Passive Transport, Actually Explained
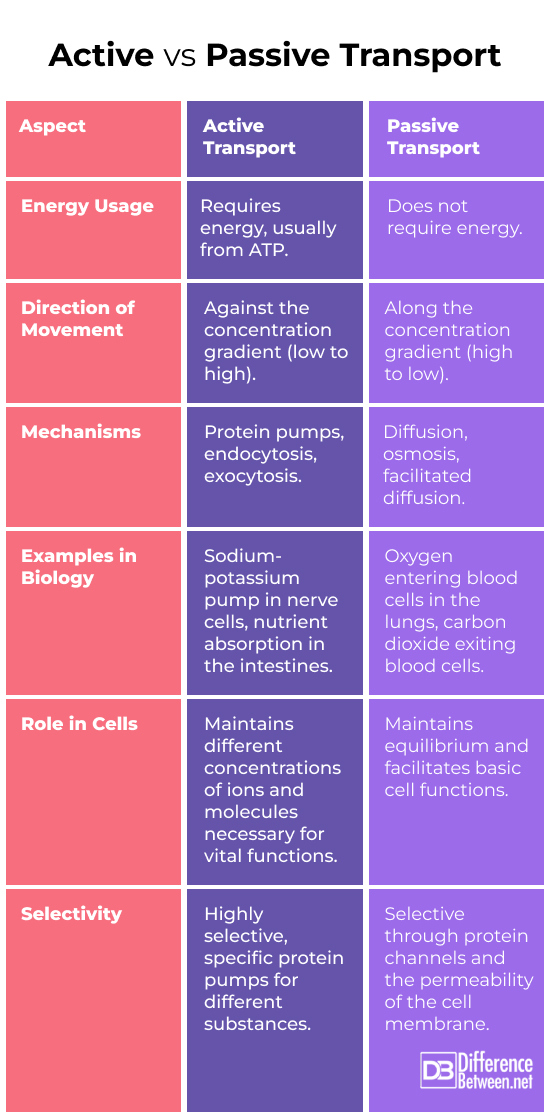
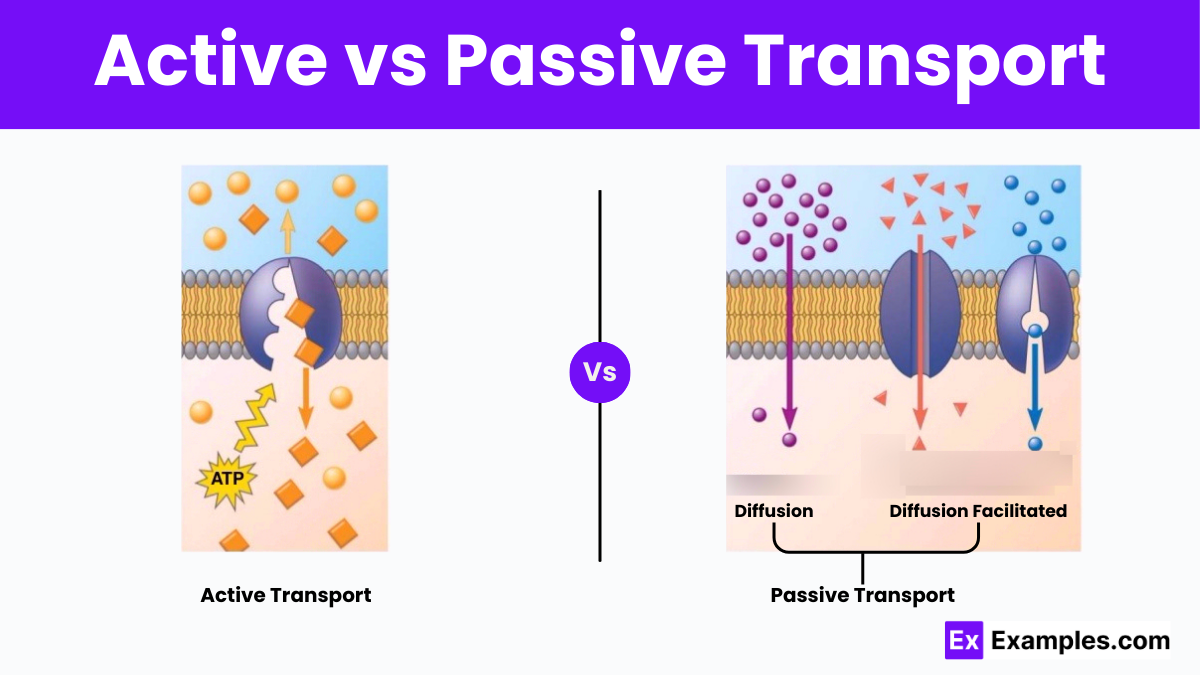
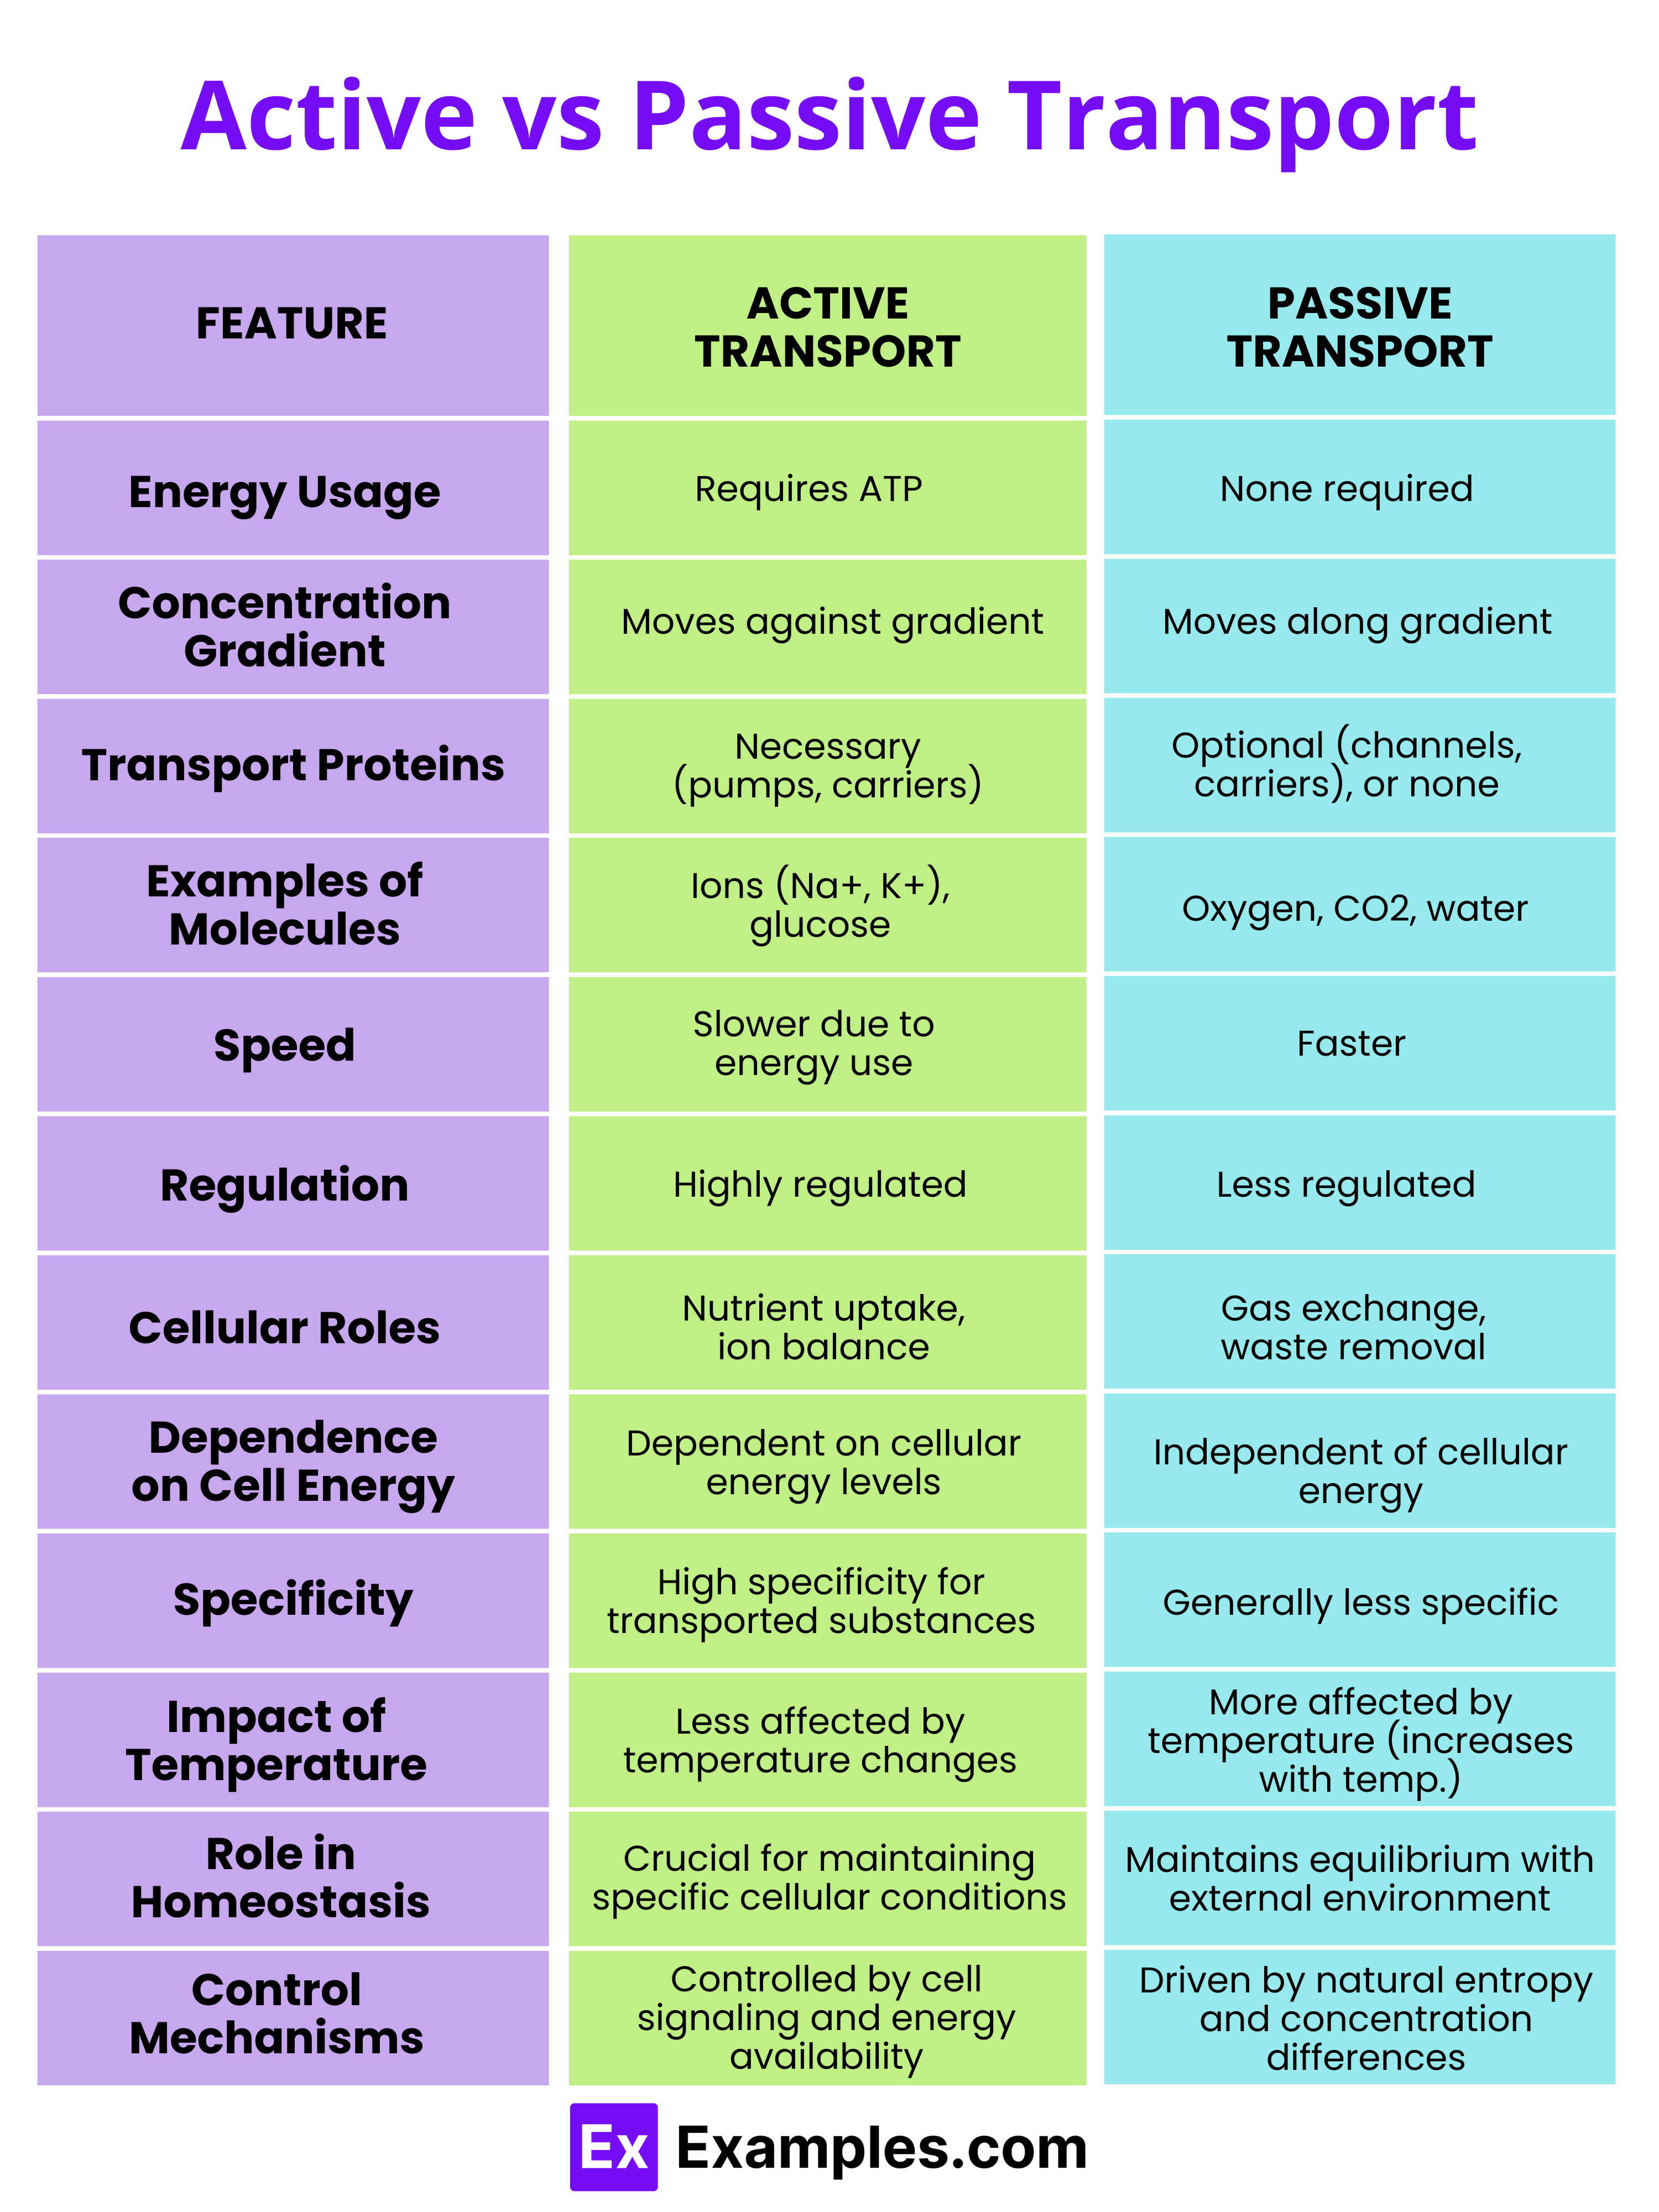
Most textbooks present this as a clean binary. It isn't. I ran into this last year when I was troubleshooting ion channel behavior in epithelial tissue cultures, and the model answer sheet kept getting it wrong.The core distinction is simple enough: passive transport moves molecules down their electrochemical gradient without expending metabolic energy. Active transport moves molecules against that gradient and requires ATP or an equivalent energy source. Where it gets messy is in the middle ground, which is where everything interesting actually lives. Passive transport includes simple diffusion, facilitated diffusion through channels or carriers, and osmosis. The sodium-potassium pump is the textbook example of primary active transport. Secondary active transport, like the sodium-glucose cotransporter SGLT1, couples the movement of one molecule against its gradient to the movement of another down its gradient. It doesn't use ATP directly, but it depends entirely on a gradient that primary active transport created and maintains. You can't classify it as purely passive without understanding the upstream energy cost. I spent a week debugging why glucose uptake in my cultured intestinal cells was far lower than expected. The assumption was that SGLT1 expression was downregulated. It wasn't. The Na+/K+ ATPase on the basolateral membrane had been inhibited by ouabain contamination in the culture medium, which collapsed the sodium gradient. Without that gradient, secondary active transport stops, even though the transporter protein itself is perfectly functional. The workaround was switching to a fresh batch of media from a different lot and running a controls assay with a known ouabain-resistant pump variant to confirm the mechanism. Took three days to isolate, two more to validate.
What people miss is that passive transport isn't just "nothing happens, stuff moves." Facilitated diffusion through carriers like GLUT1 shows saturation kinetics identical to enzyme-catalyzed reactions. The transporter has a Vmax and a Km. At high substrate concentrations, the membrane is fully occupied and the transport rate plateaus. This matters if you're doing anything quantitative, like calculating flux across a membrane in a drug delivery model. Treating facilitated diffusion as linear produces wildly inaccurate predictions once concentrations approach the transporter's affinity threshold. Another thing that trips people up: water movement. Osmosis is passive, but aquaporins aren't always necessary. Some membranes are permeable to water through the lipid bilayer itself, just much more slowly. In red blood cells, aquaporin-1 makes the difference between surviving in hypotonic solution and lysing within seconds. In the collecting duct of the kidney, vasopressin regulates how many aquaporin-2 channels get inserted into the apical membrane. That insertion process is actively regulated, but the water flowing through the channel is moving passively. The regulation is active. The transport itself is passive. The line matters more than it seems. There's also a category some people forget: vesicular transport. Endocytosis and exocytosis require ATP, so they're active. But they don't move individual molecules across the membrane in the same way ion pumps do. They move bulk material in membrane-bound containers. Pinocytosis, phagocytosis, receptor-mediated endocytosis all fall here. They're active but structurally and mechanistically distinct from pump-based transport, which can confuse people when they're comparing mechanisms side by side.
The practical implication for anyone working with cell cultures or tissue preparations: you can't isolate passive from active transport experimentally without inhibitors. Use vanadate to block P-type ATPases. Use cyanide or antimycin to collapse oxidative phosphorylation and cut off ATP production. Use gramicidin to create passive proton leaks. Each approach has artifacts. Vanadate doesn't discriminate between all P-type pumps. Cyanide affects everything that depends on mitochondrial respiration, not just your transport system. Gramicidin forms non-selective cation channels and will depolarize your membrane potential, which indirectly affects every electrogenic transporter in the cell. There is no clean experimental condition. You make the best approximation you can and account for the noise. I've seen students and researchers alike conflate concentration gradient direction with energy requirement. A molecule can move with its gradient and still require a transporter protein. That's facilitated diffusion, passive. A molecule can move against its gradient using energy from a different molecule's gradient rather than direct ATP hydrolysis. That's secondary active transport. Both are active in the sense that they involve protein-mediated directional movement. Only one directly consumes ATP. The classification depends on where the energy comes from, not on whether a protein is involved. If you're studying for an exam, memorize the pump examples and the diffusion types separately, then practice mapping them onto real tissues. Kidney proximal tubule is a good stress test because it uses both primary and secondary active transport extensively, along with passive paracellular movement, all in the same segment. Getting confused there means you haven't actually internalized the distinction yet. Working through it until it clicks is worth more time than rereading the chapter.
Get the Full Details