Most people learn this pathway by memorizing four repeating steps, but that approach falls apart the moment you try to actually apply it. I spent three semesters watching students struggle with beta oxidation when the fatty acid chain wasn't the standard even-length straight chain everyone practices with.
The Stepwise Mechanism You Actually Need To Know
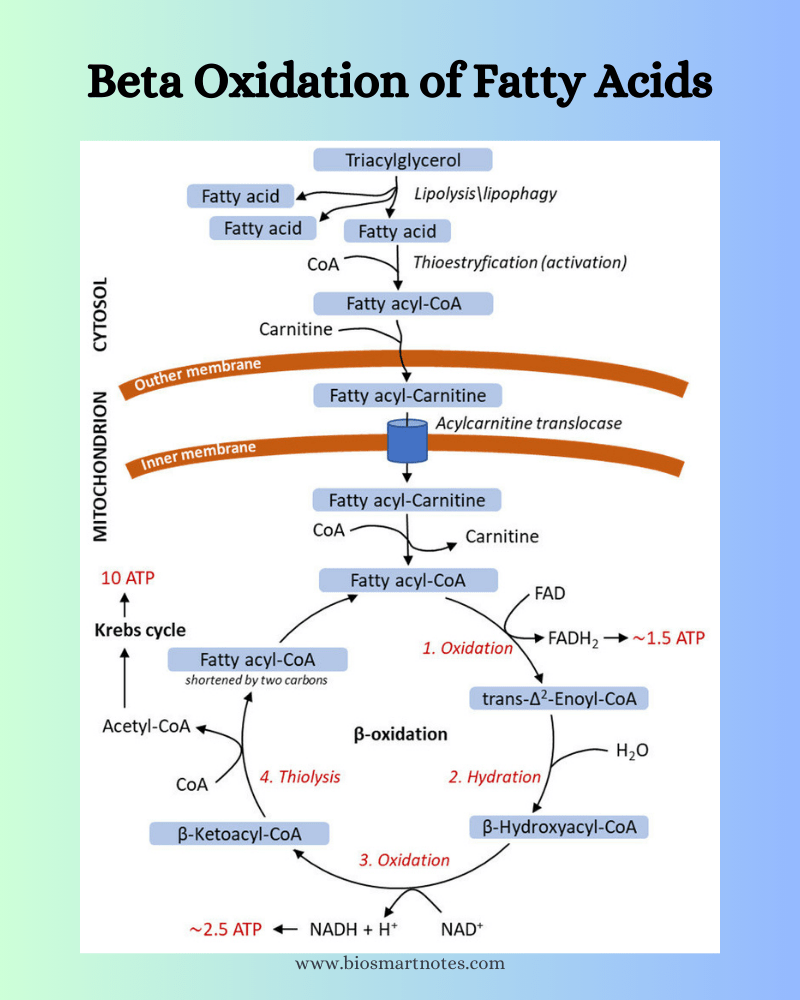
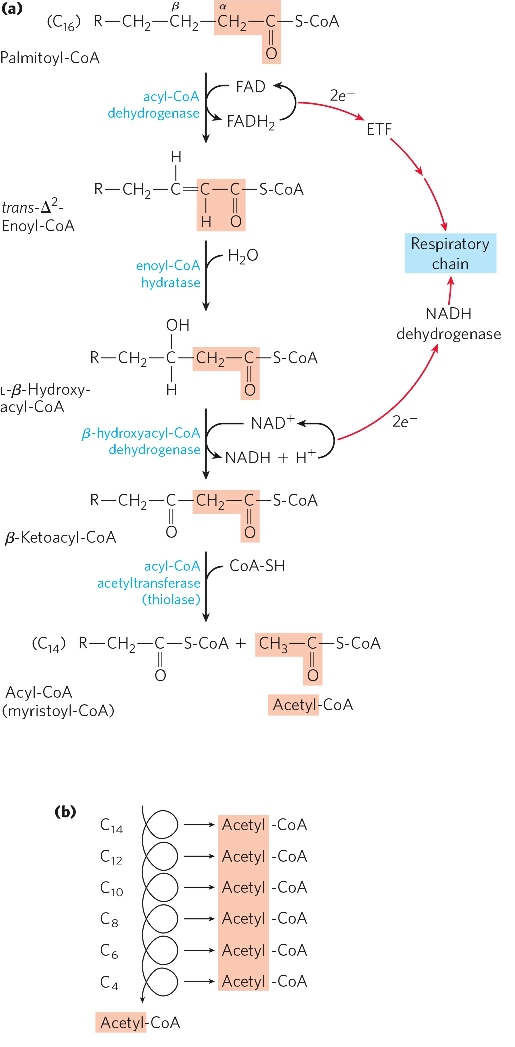
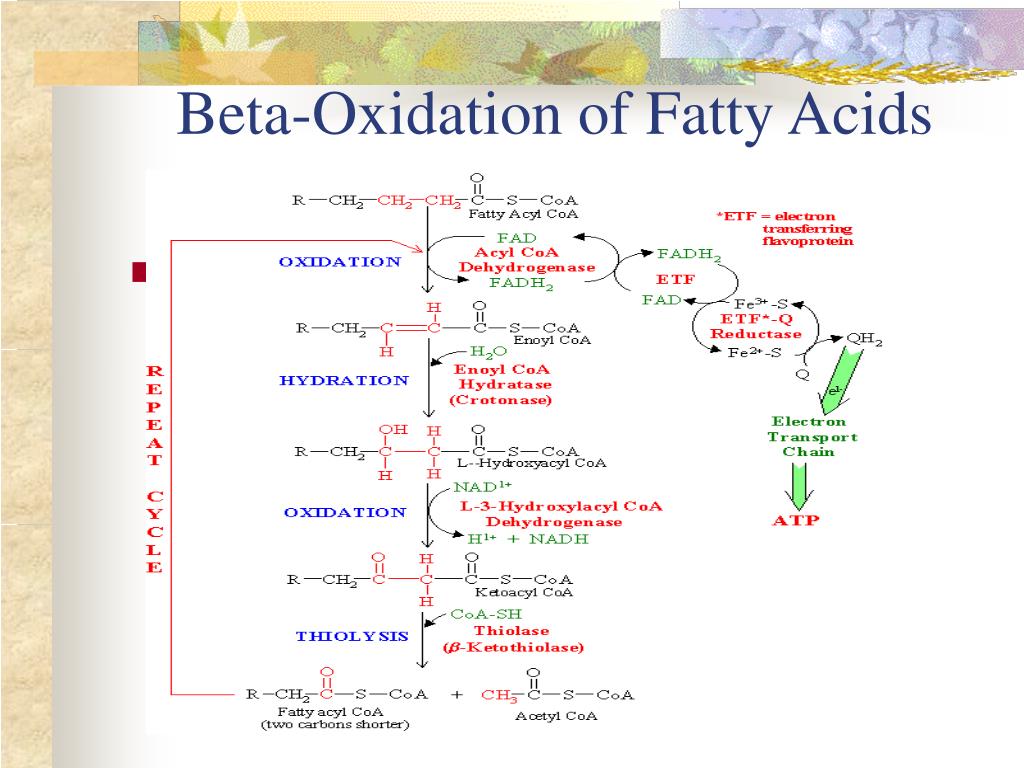
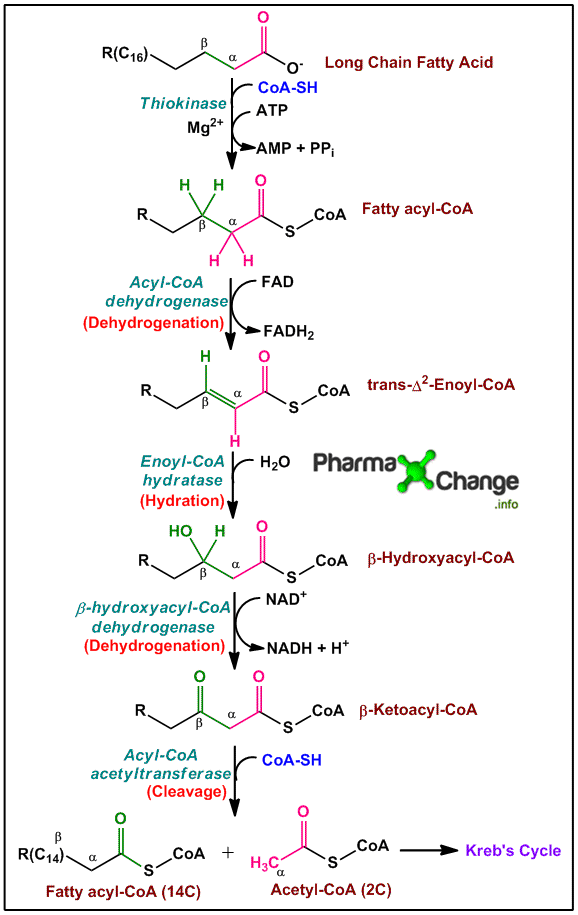
The core process strips two-carbon units from the carboxyl end of a fatty acyl-CoA through four reactions that repeat cyclically. First, an acyl-CoA dehydrogenase introduces a trans double bond between C-2 and C-3 using FAD as the electron acceptor, producing FADH2. Second, an enoyl-CoA hydratase adds water across that double bond to form L-3-hydroxyacyl-CoA. Third, a 3-hydroxyacyl-CoA dehydrogenase oxidizes the hydroxyl group using NAD+ to yield 3-ketoacyl-CoA and NADH. Fourth, thiolase cleaves off acetyl-CoA from the carboxyl side, leaving a shortened acyl-CoA that re-enters the cycle.
That is the textbook version. The actual process in a mitochondrion is messier.
Beta Oxidation Of Fatty Acids In Reality
Before any of those four steps can happen, the fatty acid has to get into the mitochondrial matrix. That requires the carnitine shuttle, and that is where most problems start in practice. Long-chain fatty acids get activated to acyl-CoA on the cytosolic side of the inner mitochondrial membrane by acyl-CoA synthetase, consuming ATP and producing AMP plus pyrophosphate. The AMP essentially counts as two high-energy phosphate bonds, so activation costs the same as breaking two ATPs to ADP.
From there, carnitine palmitoyltransferase I (CPT1) transfers the acyl group from CoA to carnitine, forming acylcarnitine. The acylcarnitine translocase shuttles it across the inner membrane in exchange for free carnitine. Once inside, CPT2 swaps the carnitine back for CoA, and the acyl-CoA is ready for beta oxidation.
The bottleneck is CPT1. It is strongly inhibited by malonyl-CoA, which is the first intermediate in fatty acid synthesis. This means when your cell is actively synthesizing fats, it simultaneously blocks their breakdown. That regulatory coupling is not optional - it is hardwired into the system.
The Edge Case That Tripped Me Up
I ran into a specific problem when modeling beta oxidation of mixed-chain substrates in a lab setting. We were tracing oxidation rates of both even-chain and odd-chain fatty acids simultaneously using isotope-labeled precursors, and the standard calculation framework kept giving inconsistent ATP yields. The issue was that odd-chain fatty acids produce propionyl-CoA instead of acetyl-CoA as the final product, and propionyl-CoA gets converted to succinyl-CoA, which enters the TCA cycle at a different point.
The workaround was straightforward but easy to miss. I had to adjust the stoichiometric accounting to reflect that propionyl-CoA carboxylase uses biotin and ATP to convert propionyl-CoA to D-methylmalonyl-CoA, then a racemase flips it to L-methylmalonyl-CoA, and methylmalonyl-CoA mutase rearranges it to succinyl-CoA using vitamin B12 as a cofactor. That B12-dependent step is a real vulnerability. If someone is B12 deficient, odd-chain fatty acid oxidation stalls at methylmalonyl-CoA, and you get methylmalonic acid accumulating in the blood. I've seen this in clinical reports more than once. The standard textbook pathway simply does not account for this.
Counter-Intuitive Details Beginners Miss
Here is something most courses gloss over: the first round of beta oxidation for a saturated even-chain fatty acid uses FAD and NAD+ but produces no GTP directly. The ATP yield comes entirely from oxidative phosphorylation downstream. For palmitate, that is 7 rounds of beta oxidation producing 7 FADH2, 7 NADH, and 8 acetyl-CoA. The acetyl-CoA feeds the TCA cycle, generating additional NADH and FADH2. The total comes to roughly 106 ATP minus 2 for activation, netting about 104 ATP per palmitate molecule.
But here is the part that catches people: this number assumes perfect coupling. In practice, the proton leak across the inner mitochondrial membrane and the cost of transporting ADP and Pi into the matrix mean the real yield is closer to 90 to 100 ATP. If you are building a metabolic model, use 96 as a realistic value rather than the theoretical maximum.
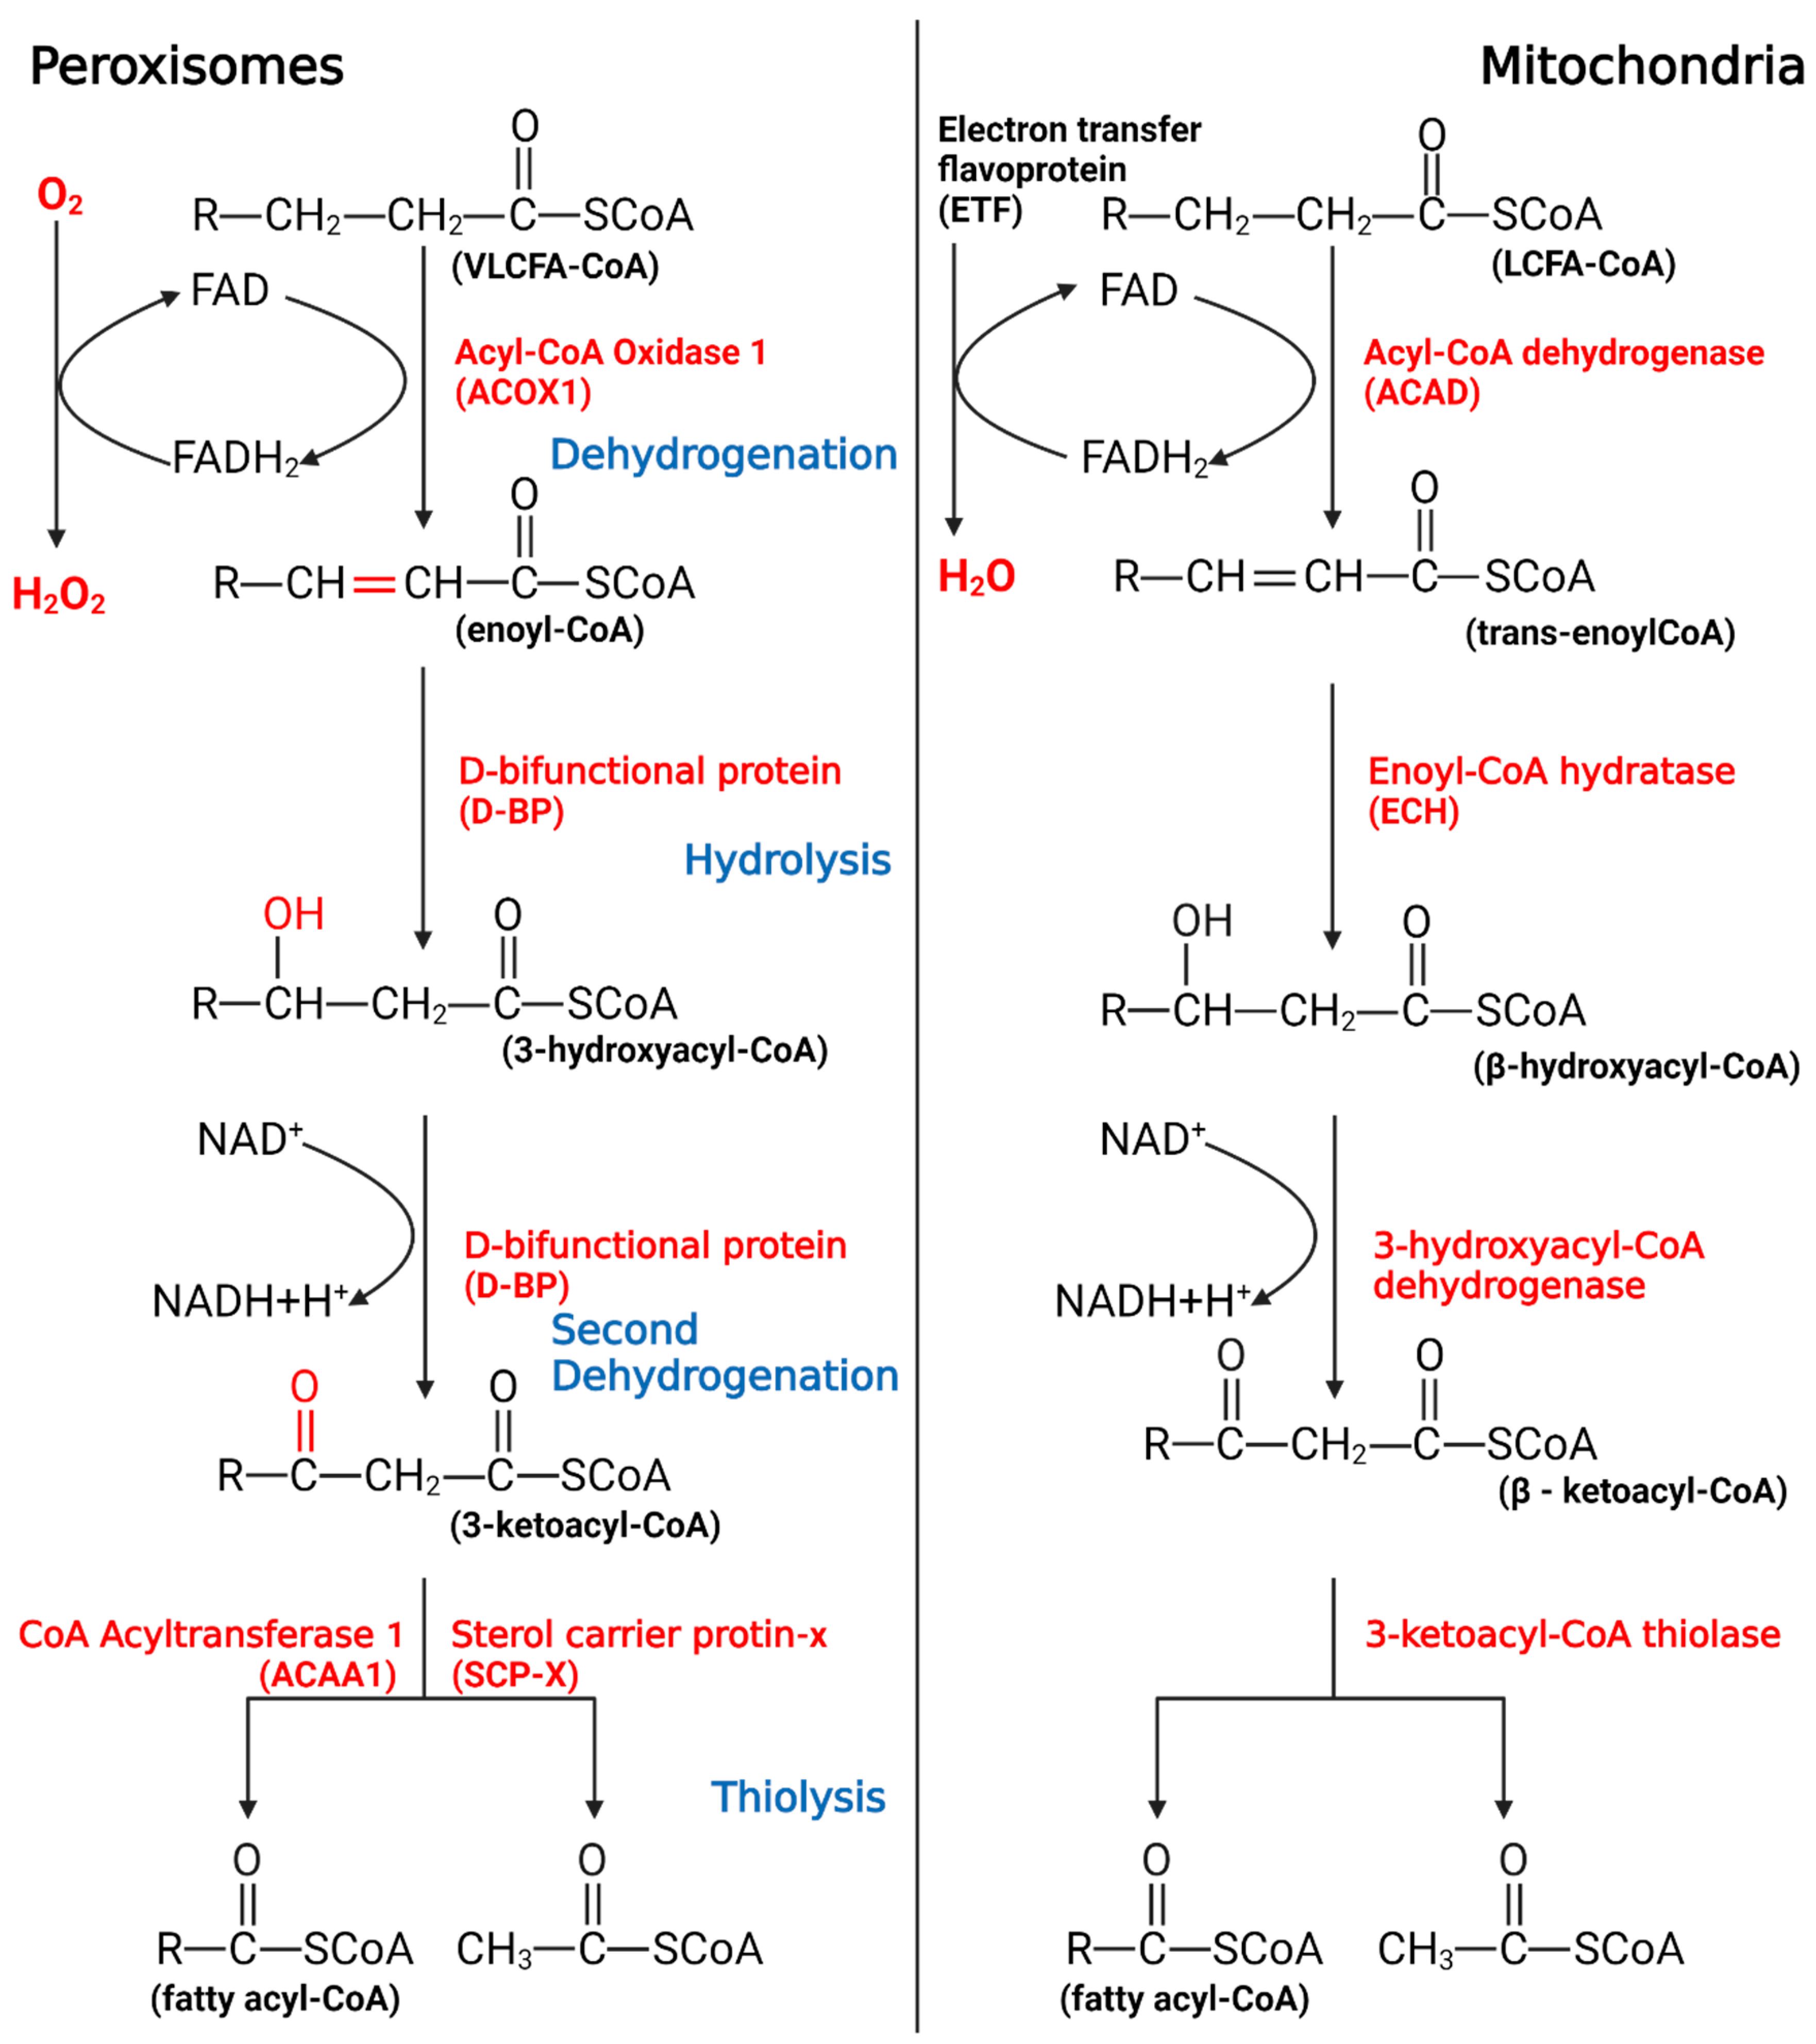
Another thing that is easy to get wrong involves the different acyl-CoA dehydrogenases. Very long-chain fatty acids are handled by VLCAD in the outer mitochondrial membrane and also in peroxisomes. Medium-chain by MCAD. Short-chain by SCAD. Each has different substrate preferences and different genetic diseases associated with their deficiency. MCAD deficiency is the most common inherited disorder of fat metabolism, affecting roughly 1 in 15,000 people in populations of European descent. During fasting, these individuals cannot oxidize medium-chain fatty acids effectively, leading to hypoketotic hypoglycemia. The standard beta oxidation pathway diagram does not warn you about this, but it is clinically significant.
Peroxisomal Beta Oxidation Is A Separate System
Peroxisomes perform beta oxidation too, but the enzymes are different and the energy capture is different. The acyl-CoA oxidase in peroxisomes passes electrons directly to oxygen, producing hydrogen peroxide rather than generating a proton gradient. The FADH2 equivalent is essentially wasted as heat. Peroxisomal beta oxidation shortens very long-chain fatty acids before they are exported to mitochondria for complete oxidation. If peroxisomal function is impaired, very long-chain fatty acids accumulate, which is exactly what happens in Zellweger spectrum disorders. The mitochondrial pathway alone cannot handle C24 and longer chains efficiently.
A Note On Unsaturated Fatty Acids
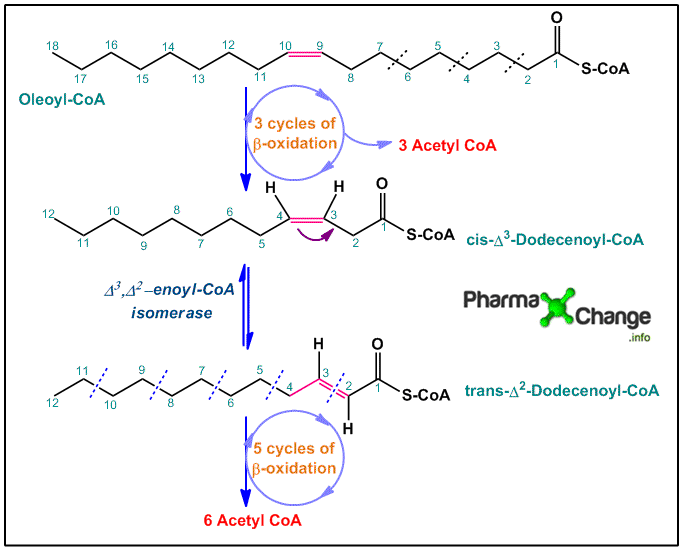
Unsaturated fatty acids require two extra enzymes because the natural beta oxidation machinery only handles trans-delta-2 double bonds. Cis-delta-9 double bonds in oleate, for example, need an isomerase after the first round to shift the bond into the right configuration. cis,cis-Delta-6 double bonds in linoleate need both an isomerase and a reductase because the reductase uses NADH to saturate an extra double bond before the isomerase can reposition it. These extra steps consume reducing equivalents, so the ATP yield from unsaturated fatty acids is lower than the textbook calculation suggests. I have seen graduate students forget to account for the NADH consumed by the 2,4-dienoyl-CoA reductase step when computing yields from arachidonic acid oxidation.
Practical Modeling Approach
If you are building a computational model of fatty acid oxidation, I recommend starting with the stoichiometric matrix for the core four-step cycle and then adding branches for chain length, saturation state, and compartmentalization. The carnitine shuttle should be modeled as a reversible transport step with CPT1 as the regulated node. Use malonyl-CoA concentration as the inhibitory signal on CPT1 rather than hard-coding the inhibition. This makes the model responsive to nutritional state changes.
For substrate-specific yields, do not rely on a single formula. Odd-chain and unsaturated fatty acids deviate enough that a one-size-fits-all calculation will introduce systematic error. Build in conditional logic that checks chain length and double bond positions before applying the stoichiometry.
The full substrate-level accounting for a generic even-chain saturated fatty acid with n carbons requires n/2 minus 1 rounds of beta oxidation, producing n/2 acetyl-CoA molecules, n/2 minus 1 FADH2 molecules, and n/2 minus 1 NADH molecules. Multiply the FADH2 by roughly 1.5 ATP each and the NADH by roughly 2.5 ATP each, subtract the activation cost of 2 ATP equivalents, and you have your net yield. Adjust downward by about 10 to 15 percent for physiological inefficiency.
Gallery Beta Oxidation Of Fatty Acids
Beta Oxidation Of Fatty Acids Khan Academy – SVWWW
Beta Oxidation Of Fatty Acids Quizlet at Yi Voss blog
Beta Oxidation Of Polyunsaturated Fatty Acids – HQCWDZ
Fatty Acids Undergo Beta Oxidation at Rosalind Rinaldi blog
Beta-oxidation of Fatty Acid