Getting past the textbook definition and actually using coevolution as an analytical tool
The Biology Definition Of Coevolution describes reciprocal evolutionary change between two or more interacting species, where each exerts selective pressure on the other. That is the one-sentence version you find in introductory courses. It is also almost useless for anything beyond a basic quiz. The concept gets mangled frequently because people treat it as a neat little package when in reality the patterns in the wild are messy, asymmetrical, and often involve more than two players even when you are only tracking two. I spent years working on host-parasite systems and trying to determine whether an observed trait shift in one species was truly the result of coevolution or just a side effect of environmental change. The distinction matters because your methodology changes entirely depending on which one you are dealing with. Coevolution requires evidence that the interaction is reciprocal. You need to show species A evolved a trait in response to species B, and species B evolved a trait in response to species A. Without both arms of that loop, you do not have coevolution. You have something else, and calling it coevolution just sounds impressive. The standard approach involves phylogenetic comparison. You build trees for both organisms and look for congruence. If the host tree and the parasite tree mirror each other, that is a strong signal of co-speciation, which is one type of coevolutionary outcome. But congruence alone does not prove coevolution. It could mean both lineages responded to the same geographic isolation events. You need to rule out vicariance before you claim the organisms drove each other evolutionarily.
One practical method I rely on is the geographic mosaic theory framework. Coevolution is not uniform across a species range. There are coevolution hotspots where the reciprocal selection is intense, and there are coldspots where the interaction has faded or reversed direction. Mapping these mosaics takes effort. You need population-level genetic data across multiple contact zones, plus phenotypic measurements from the same locations. I once spent six field seasons sampling a plant-herbivore system across a forty kilometer transect before the mosaic pattern became clear enough to publish anything useful. If you want a more quantitative handle on it, consider using reciprocal transplant experiments or common garden setups. Place individuals from different populations into each other's environments and measure fitness components directly. When a plant from population A grows better on its local herbivore than on the foreign one, and the herbivore from population A performs worse on the foreign plant, that is localized adaptation consistent with coevolution. It does not prove reciprocity on its own, but combined with phylogenetic data it strengthens the case considerably.
Common pitfalls that waste time and resources
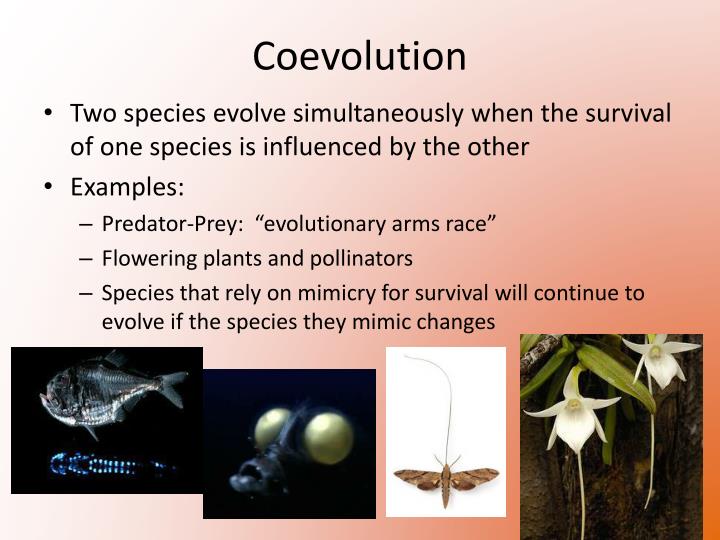
The most frequent mistake I see is assuming that trait matching equals coevolution. A flower with a long corolla and a moth with a long proboscis look like a textbook chase. They might be. They might also be responding to completely different selective forces. The flower could be adapting to a pollinator that is not the long-tongued moth at all, while the moth is simply constrained by biomechanics rather than evolutionary escalation. Trait matching without mechanistic evidence is anecdotal at best. Another problem is the time scale. Coevolutionary processes can operate over thousands to millions of years. Most researchers do not have access to that kind of temporal resolution. Fossil records rarely preserve the soft tissue interactions needed to reconstruct arms races directly. Molecular clocks help but introduce their own uncertainties. If you are studying a system where the interaction is evolutionarily recent, you may be observing the early stages of adaptation rather than an established coevolutionary dynamic. Distinguishing between the two requires dense sampling and a clear understanding of the system's history. I encountered a specific edge case involving a mycorrhizal fungus and its host plant. The fungal community shifted dramatically after the introduction of a non-native plant species nearby. The native plant showed reduced fitness, and the fungal genotype frequencies changed in response. At first glance, this looked like indirect coevolution through a shared mutualist network. But when I ran a controlled experiment removing the fungal component entirely, the native plant performed just as poorly in the presence of the invader. The real driver was resource competition, not reciprocal selection through the fungus. The fungus was a bystander that happened to track the plant community shift. I had to rewrite three chapters of a manuscript based on this finding, and it took about four months of additional greenhouse work to confirm the interpretation before I could submit again.
Get the Full Details

When coevolution models break down
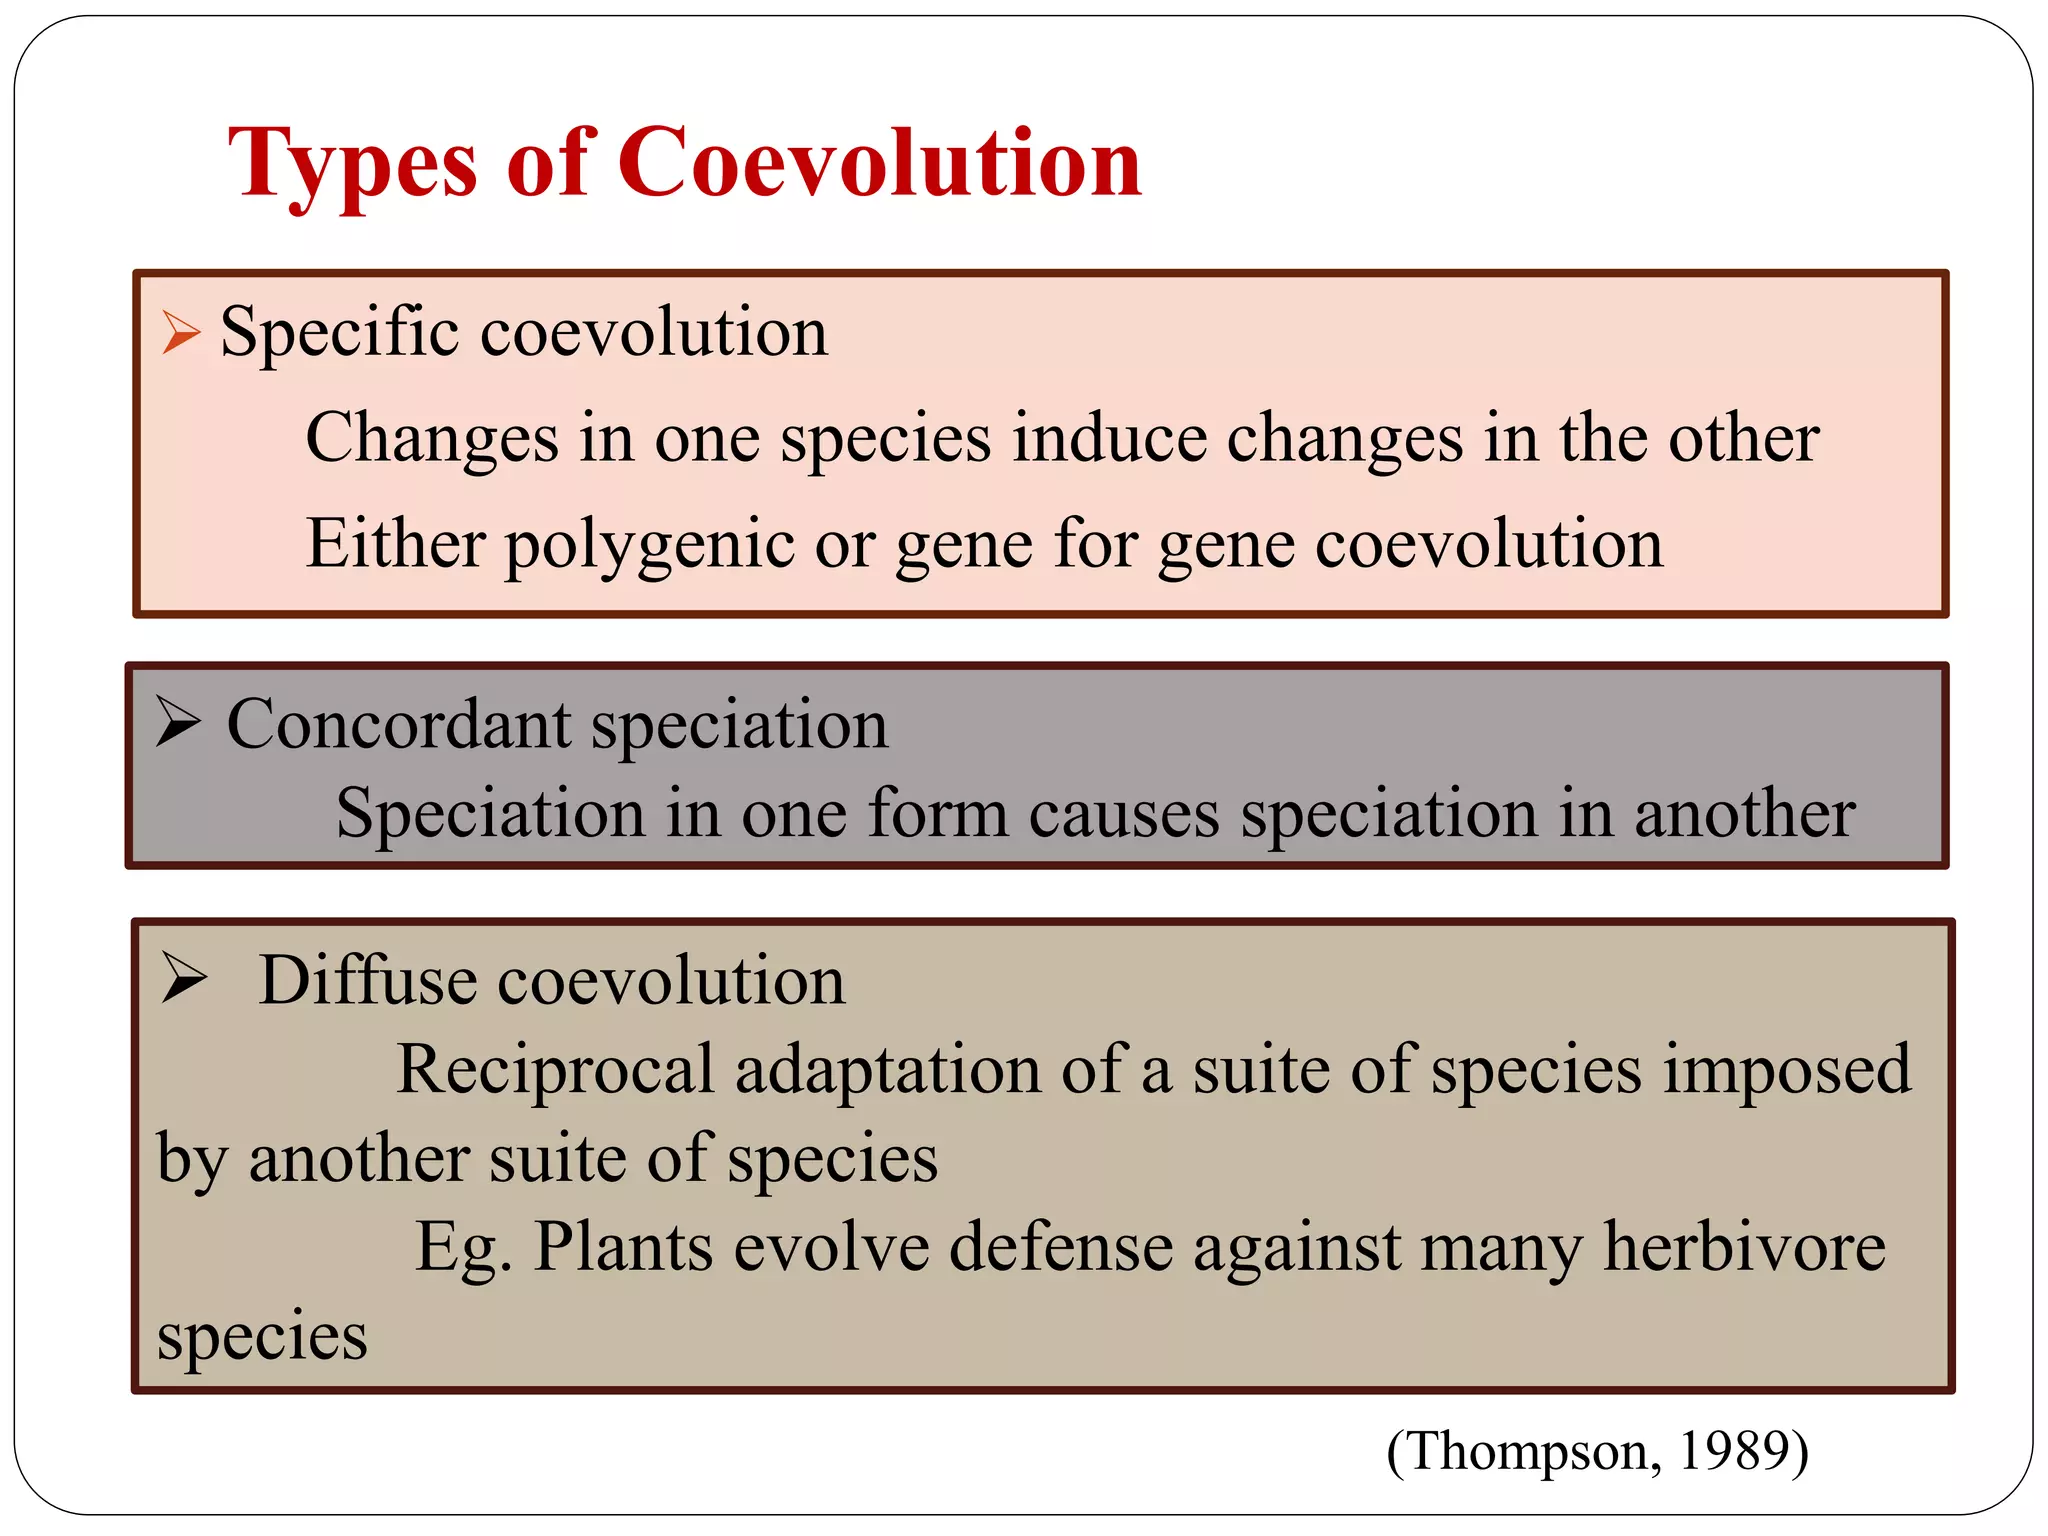
Red Queen dynamics, named after the character who said it takes all the running you can do to stay in the same place, describe a scenario where species must continuously adapt just to maintain their relative fitness. This is a powerful model for host-parasite coevolution and for sexual reproduction evolution. But it assumes constant reciprocal selection pressure. In reality, selection pressures fluctuate. Environmental variation can swamp biotic interactions. A predator-prey system that looks like a classic arms race in a stable environment may look nothing like that when drought or temperature shifts alter population densities dramatically. The Red Queen model still applies qualitatively, but the predictive power drops substantially when you cannot separate climate-driven selection from interaction-driven selection. Diffuse coevolution is another term you will encounter, referring to selection among groups of species rather than pairwise interactions. An example is a plant evolving defenses against a guild of herbivores rather than a single species. This is arguably more realistic than the pairwise model, but it is also far harder to study rigorously. The number of variables multiplies quickly, and statistical power becomes a serious constraint. Most diffuse coevolution studies rely on correlational data, which leaves them vulnerable to the same confounding factors that plague pairwise studies. If your goal is to demonstrate coevolution for a paper or grant application, the strongest evidence comes from combining multiple independent lines of inquiry. Phylogenetic congruence with vicariance ruled out, reciprocal selection demonstrated in common garden or reciprocal transplant experiments, and mechanistic understanding of how the traits interact functionally. No single line of evidence is sufficient on its own, and reviewers who know the literature will tell you that plainly.
The Biology Definition Of Coevolution remains a useful anchor point for framing questions, but the actual work of establishing coevolutionary relationships demands more than a definition. It requires systematic elimination of alternative explanations and a willingness to accept that some systems simply do not fit the clean narratives that textbooks present.