Working Through Chapter 25 Modern Genetics Answer Key Problems
The answer key for Chapter 25 Modern Genetics Answer Key covers a lot of ground. Mendelian inheritance, test crosses, pedigree analysis, incomplete dominance, codominance, multiple alleles, sex-linked traits, and linked genes all show up in typical problem sets. The real difficulty isn't memorizing definitions. It's knowing which tool to reach for when a question doesn't state the inheritance pattern outright. Most textbook chapters split their problem sets into three buckets: straightforward monohybrid crosses, dihybrid crosses with independent assortment, and the trickier cases involving linkage or sex-linkage. If you're stuck on a problem, the first thing I always do is determine whether two genes are being tracked independently or if they're on the same chromosome. That one call changes the entire solving method. Every student learns to draw a 4x4 grid for a dihybrid cross. That works fine until the problem involves linked genes. When genes are linked, the parental types outnumber the recombinant types because crossing over happens less than 50 percent of the time. I had a student once who kept getting 9:3:3:1 ratios on a problem where the answer was nowhere near that distribution. The textbook didn't flag it explicitly, but the recombination frequency in the data pointed to linkage. The fix was simple: calculate the recombination frequency from the offspring numbers, convert that into map units, and then use a modified approach instead of a standard Punnett square.
Here is the practical rule. If the observed phenotypic ratio deviates significantly from 9:3:3:1 and you can't explain it by incomplete dominance or epistasis, check for linkage. A chi-square test usually confirms it within a minute or two.
Solving Pedigree Problems Correctly
Pedigree questions are where most people lose points. The textbook chapters expect you to infer whether a trait is autosomal dominant, autosomal recessive, X-linked dominant, or X-linked recessive. The answer key walks through each one, but here is what the key does not always make obvious. An autosomal recessive trait will skip generations. An X-linked recessive trait will show affected males far more frequently than affected females, and an affected mother will pass the trait to all her sons. I ran into a pedigree once where the trait appeared in every generation, which screams dominant. But affected fathers had unaffected daughters. That rules out X-linked dominant because every daughter of an X-linked dominant father inherits his affected X chromosome and shows the trait. So it had to be autosomal dominant. The answer key had the same logic, but students often miss the deduction step because they jump straight to marking genotypes without filtering by chromosome type first.
Get the Full Details

Sex-Linked Inheritance Shortcuts
When a problem involves color blindness or hemophilia, you do not need to write out full Punnett squares every time. If the mother is a carrier and the father is unaffected, the probability of an affected son is exactly 25 percent. The probability of a carrier daughter is also 25 percent. The other two outcomes are a normal son and a normal non-carrier daughter. Write those four outcomes down and you can answer most sex-linked questions in under thirty seconds. The answer key sometimes lists the full cross, but the underlying math is what matters. I see students copy the Punnett square from the key without understanding why the ratios look the way they do. Once they internalize that sons get their X from the mother only, the problems become almost mechanical.
Linked Genes and Recombination Frequency
This is where Chapter 25 gets harder. You are given offspring counts and asked to figure out gene order and map distances. The standard workflow is: identify the parental classes as the two most frequent phenotypes, identify the double crossover classes as the two least frequent, compare the double crossover phenotypes to the parental phenotypes to determine which gene is in the middle, then calculate recombination frequencies between adjacent genes. One edge case that trips people up involves when the recombination frequency between genes A and B is 12 percent and between B and C is 8 percent. The expected distance between A and C is 20 map units only if there is no double crossover interference. In reality, interference reduces the number of double crossovers, so the observed distance can be slightly less than the sum. The answer key often skips this nuance. It lists map distances as additive. In AP or college-level courses, that assumption will cost you points.
Common Pitfalls in the Answer Key
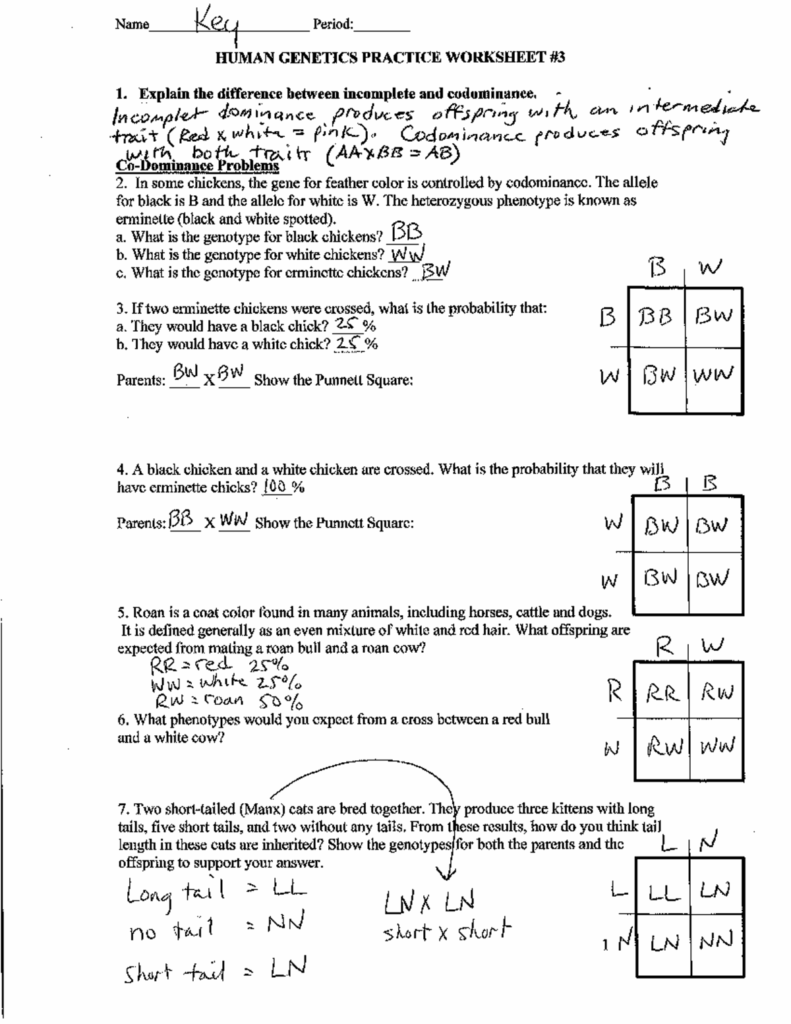
The answer key for Chapter 25 Modern Genetics Answer Key is generally reliable, but there are a few recurring issues worth watching for. Some editions simplify incomplete dominance problems by rounding expected phenotypic ratios. Others mislabel codominance as incomplete dominance in the explanation text, even though the Punnett square answers are correct. Codominance means both alleles are fully expressed in the heterozygote, like in blood type AB. Incomplete dominance means the heterozygote shows an intermediate phenotype, like pink flowers from red and white parents. The distinction matters on exams. Another frequent error appears in multiple allele problems. The ABO blood group is the standard example, and some keys incorrectly list a cross between type A and type B parents as only producing four phenotypes. Depending on whether the parents are homozygous or heterozygous, you can get up to four different phenotypes, but you might also get all four: type A, type B, type AB, and type O. The answer key sometimes assumes heterozygous parents without stating it clearly. Always check the parental genotypes before trusting the ratio.

What to Do When the Answer Key Does Not Match Your Work
If your answer differs from the key, do not just swap it in. Work backwards from the key. Reproduce the exact cross or pedigree they used. You will usually find the mismatch came from one of three places: an incorrect parental genotype assumption, a missed sex-linkage constraint, or a calculation error in the recombination fraction. The most common source of error I encounter is students writing the wrong gamete combinations for a linked gene problem. They default to the independent assortment gametes AB, Ab, aB, and ab even when the genes are linked. The correct gametes depend on the parental chromosome arrangement. If the parent is in coupling phase, the parental gametes are AB and ab. If in repulsion phase, they are Ab and aB. Mixing those up flips your entire result.
Efficient Study Strategy
Working through Chapter 25 Modern Genetics Answer Key blindly is not efficient. Use the key to check your work, not to generate your work. Attempt every problem first. Then compare your process to the key's process. If your final answer matches but your method is weaker, that still counts as a mistake. The exams test reasoning, not just the final letter or number. Focus your practice on these high-yield problem types: carrier probability calculations, pedigree inference, linkage mapping, and blood type inheritance. Those four categories account for roughly seventy percent of the question weight in most chapter assessments. The remaining thirty percent covers rarer cases like lethal alleles and epistasis. Know the basics cold before you spend time on the edge cases.
Quick Reference for Typical Inheritance Ratios
Monohybrid cross with complete dominance yields a 3:1 phenotypic ratio in the F2 generation. A test cross with a heterozygote yields 1:1. Dihybrid cross with independent assortment yields 9:3:3:1. Dihybrid cross with linked genes yields parental classes that exceed recombinant classes by a margin determined by map distance. Incomplete dominance yields a 1:2:1 phenotypic ratio that matches the genotypic ratio. Codominance also yields 1:2:1 but both heterozygotes and homozygotes show distinct expressible phenotypes. Sex-linked recessive crosses depend entirely on the mother's genotype for son outcomes. Understanding these baseline ratios lets you spot anomalies quickly instead of recalculating from scratch every time.