What Carbon Actually Does in Biological Systems
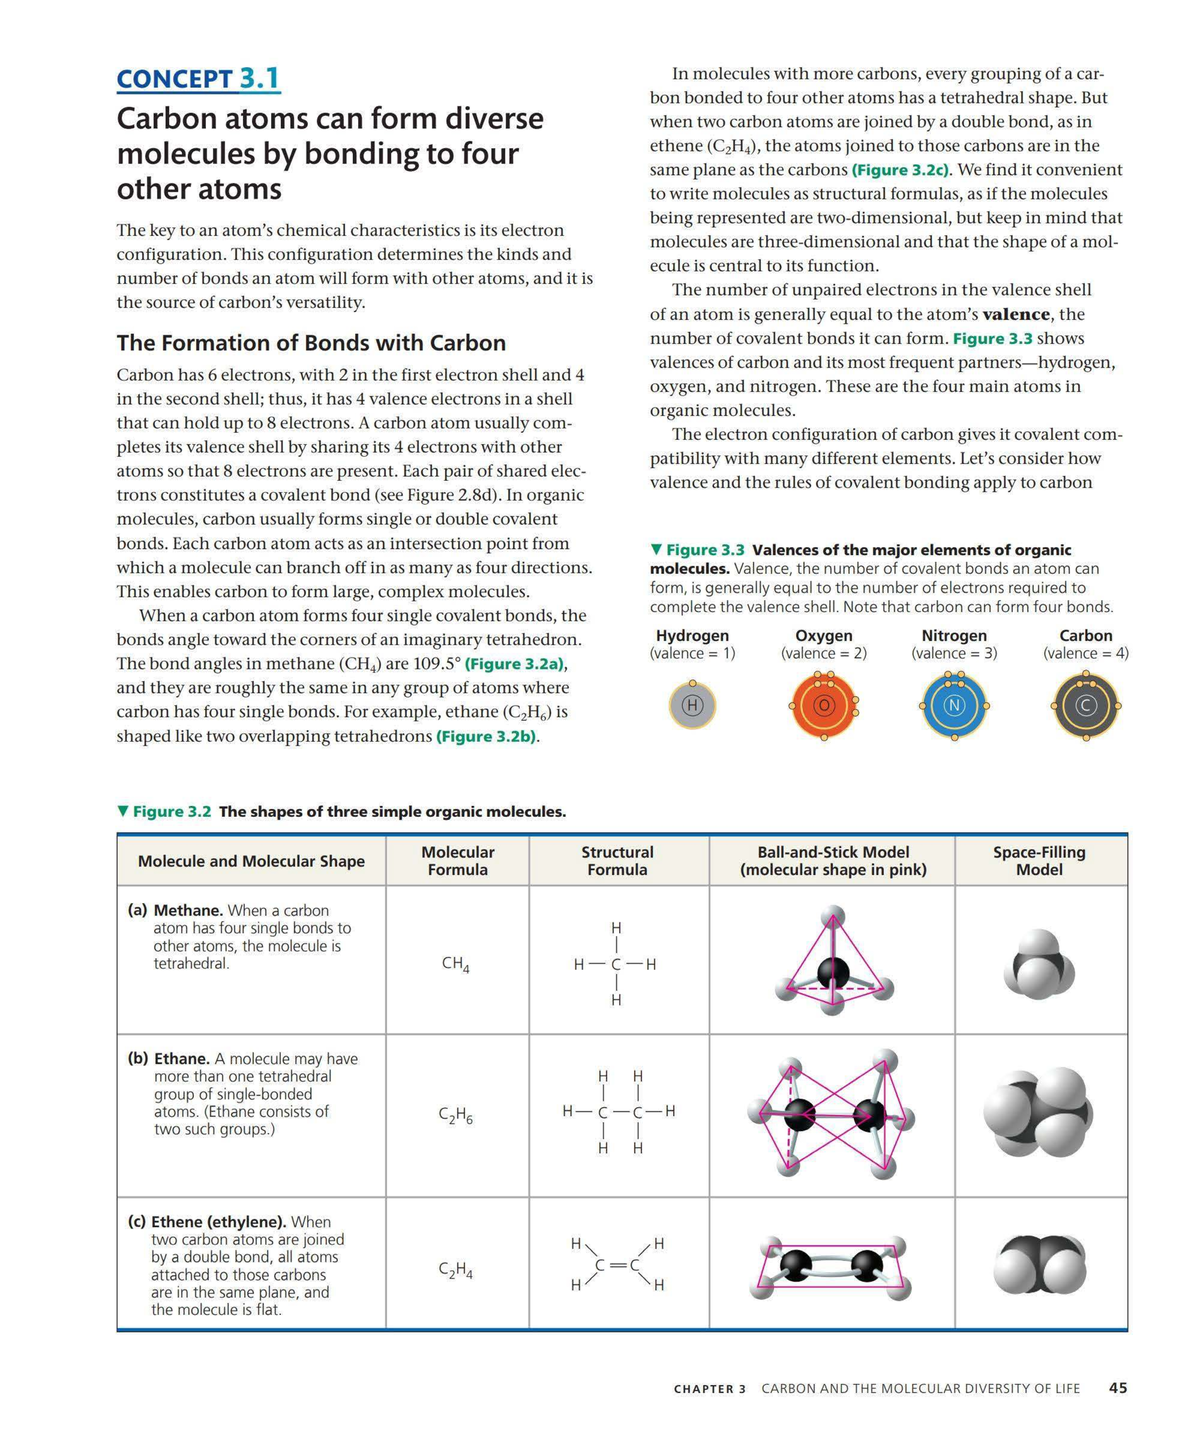
Carbon forms four covalent bonds because of its electron configuration. That single fact—tetravalence—is the reason organic molecules exist in such vast numbers. You can arrange four bonds in different spatial configurations, connect carbons to other carbons in chains or rings, and attach different functional groups to change reactivity. The variety isn't accidental. It's a direct consequence of carbon's bonding geometry.Chapter 3 Carbon And The Molecular Diversity Of Life
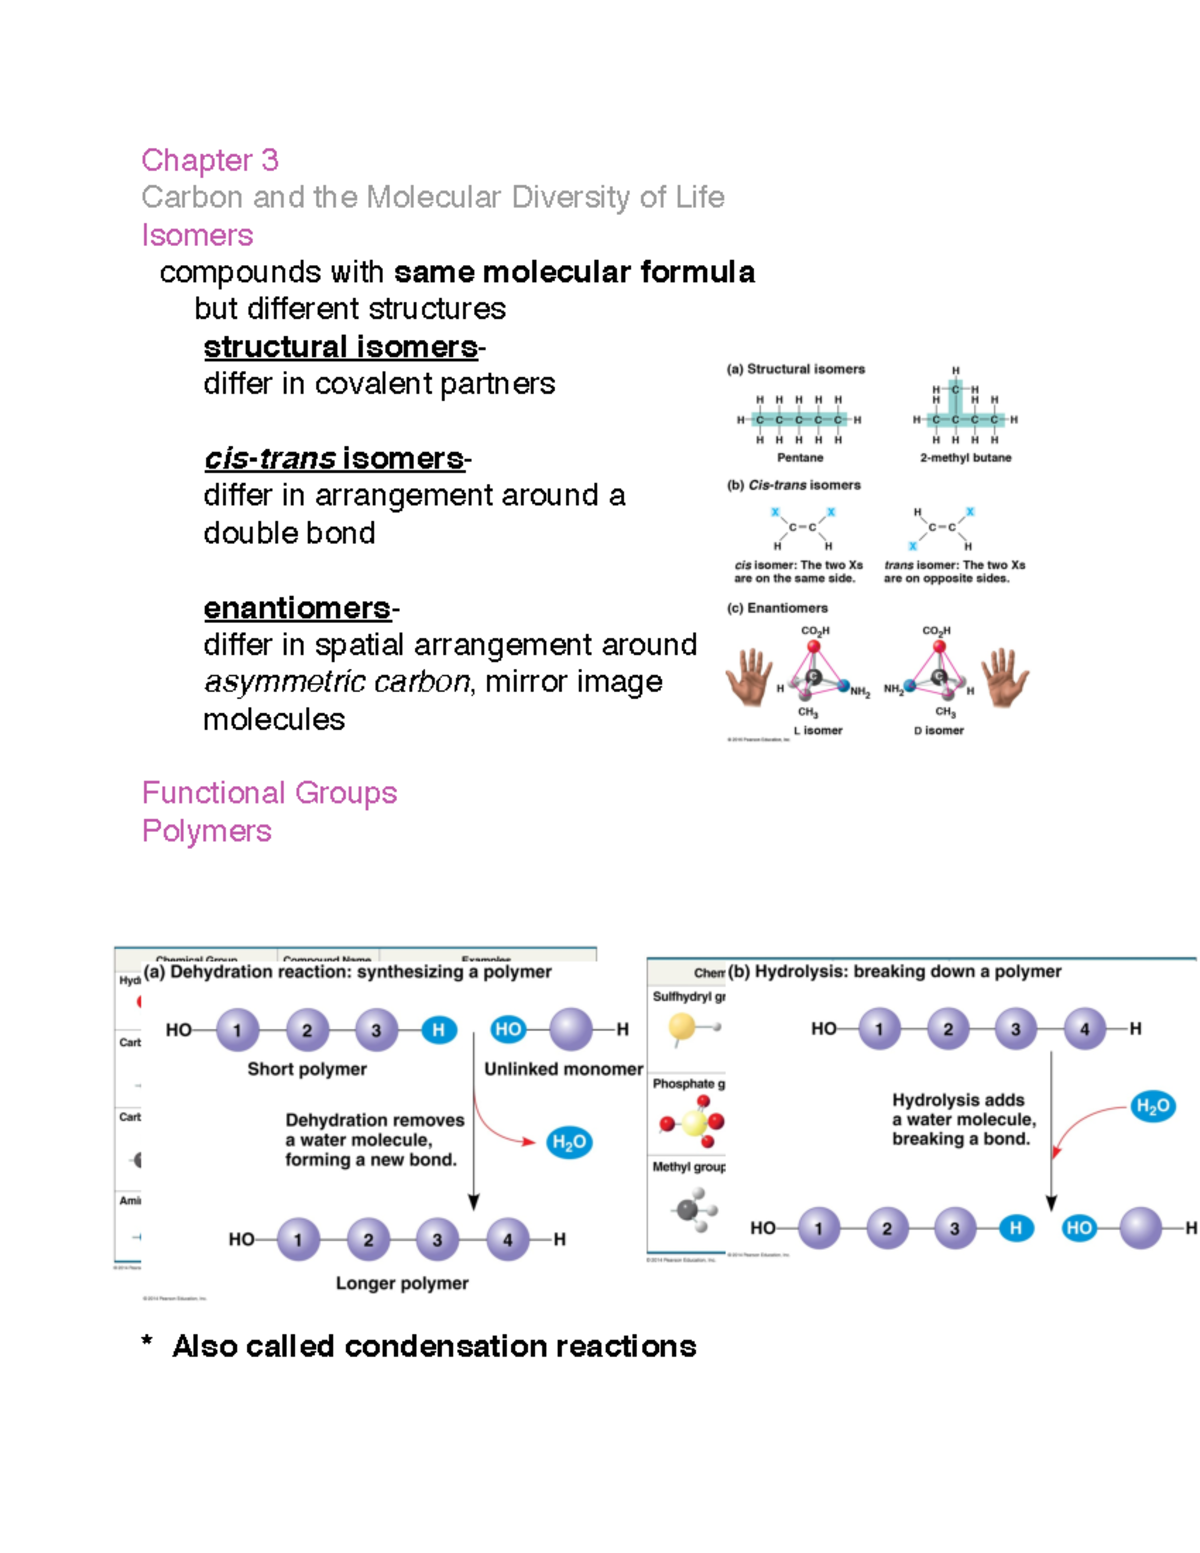
The chapter tracks how simple carbon compounds build into the polymers that make up cells. What makes this material stick is understanding isomerism and functional groups. These are the concepts that separate students who get it from those who drown in memorization. Structural isomers share a molecular formula but differ in covalent arrangement. CH can be butane—a straight chain—or isobutane, with a branched structure. They have different boiling points, different reactivities. They are not interchangeable in any biological context. Stereoisomers are where things get messier. Enantiomers are mirror-image isomers. A carbon atom bonded to four different groups creates a chiral center, and your body treats each enantiomer differently. Thalidomide is the case study everyone gets assigned. One enantiomer suppresses morning sickness. The other caused severe birth defects. Your liver's enzymes cannot distinguish between them reliably once they're in circulation. Geometric isomers are another category. Cis and trans configurations around a double bond produce molecules with different shapes and different physical properties. Phospholipid membranes depend on this. Saturated fats pack tightly because their hydrocarbon tails are straight. Unsaturated fats with cis double bonds introduce kinks that prevent tight packing. That's why olive oil is liquid at room temperature and butter is solid. The difference is a single bond geometry.
Functional Groups: The Part That Actually Matters
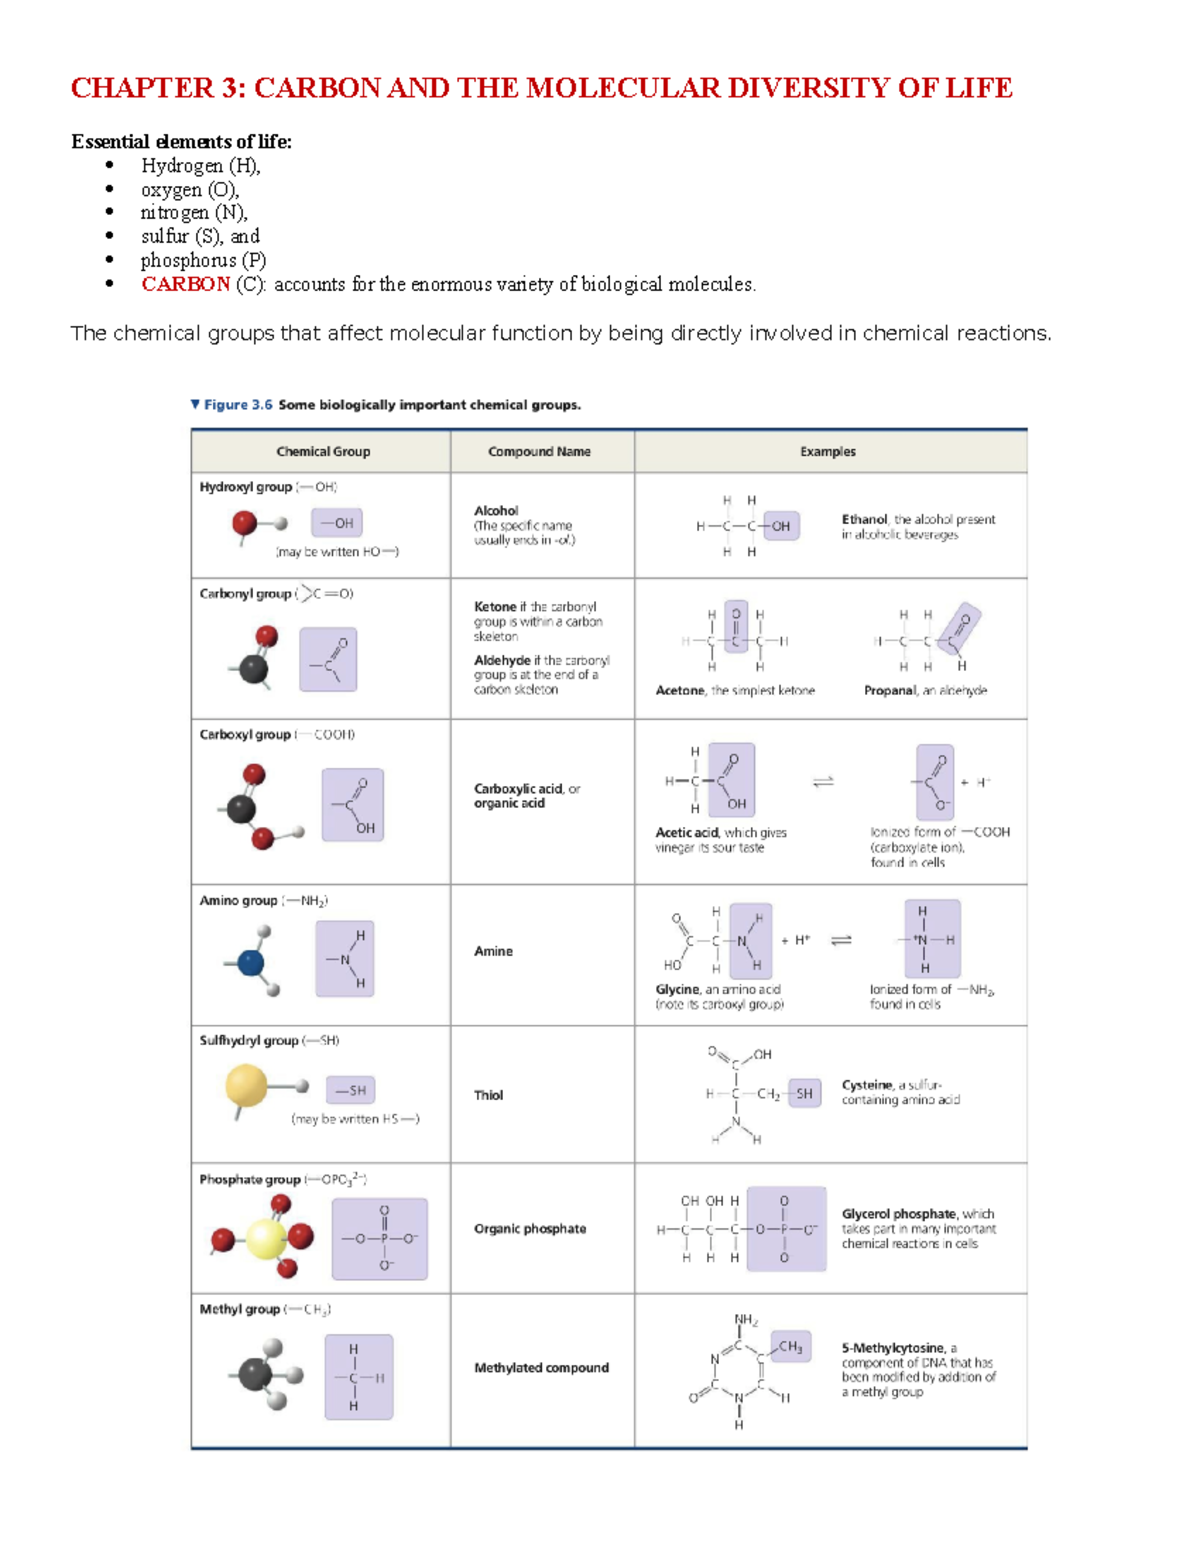
You need to know these by heart. Not the names alone, but what each group does chemically and which biological molecules contain them. Hydroxyl groups (-OH) make molecules polar and capable of hydrogen bonding. Carbonyl groups (C=O) appear in ketones and aldehydes—glucose and fructose are structural isomers that differ in carbonyl position. Carboxyl groups (-COOH) act as acids, donating protons in solution. Amino groups (-NH) act as bases. Sulfhydryl groups (-SH) form disulfide bridges that stabilize protein tertiary structure. Phosphate groups carry negative charge and are central to energy transfer through ATP. Methyl groups (-CH) are nonpolar and affect gene expression when added to DNA. I used to teach this material by having students draw functional groups repeatedly. It works better to connect each group to a real molecule you already know. Hydroxyl: ethanol, serine, glucose. Carboxyl: acetic acid, any amino acid. Phosphate: ATP, DNA backbone, phospholipids. The connections make the groups memorable without requiring rote repetition.
Polymers and the Dehydration/Hydrolysis Cycle
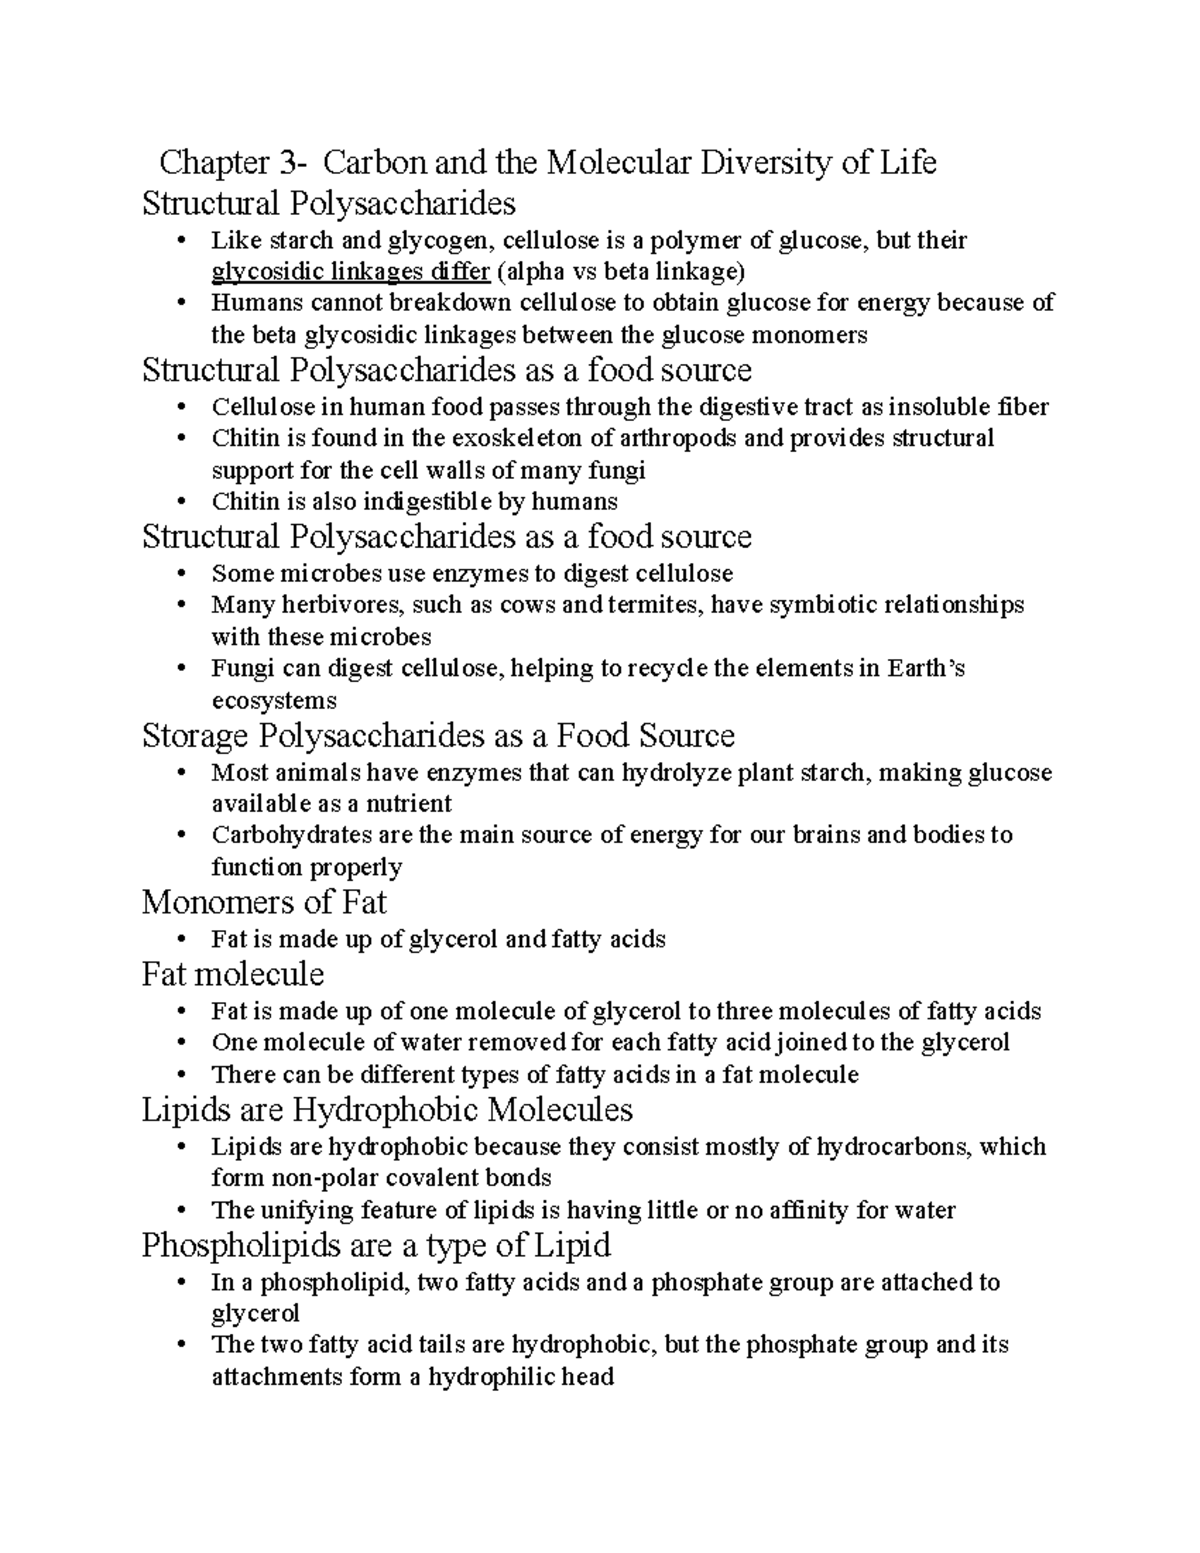
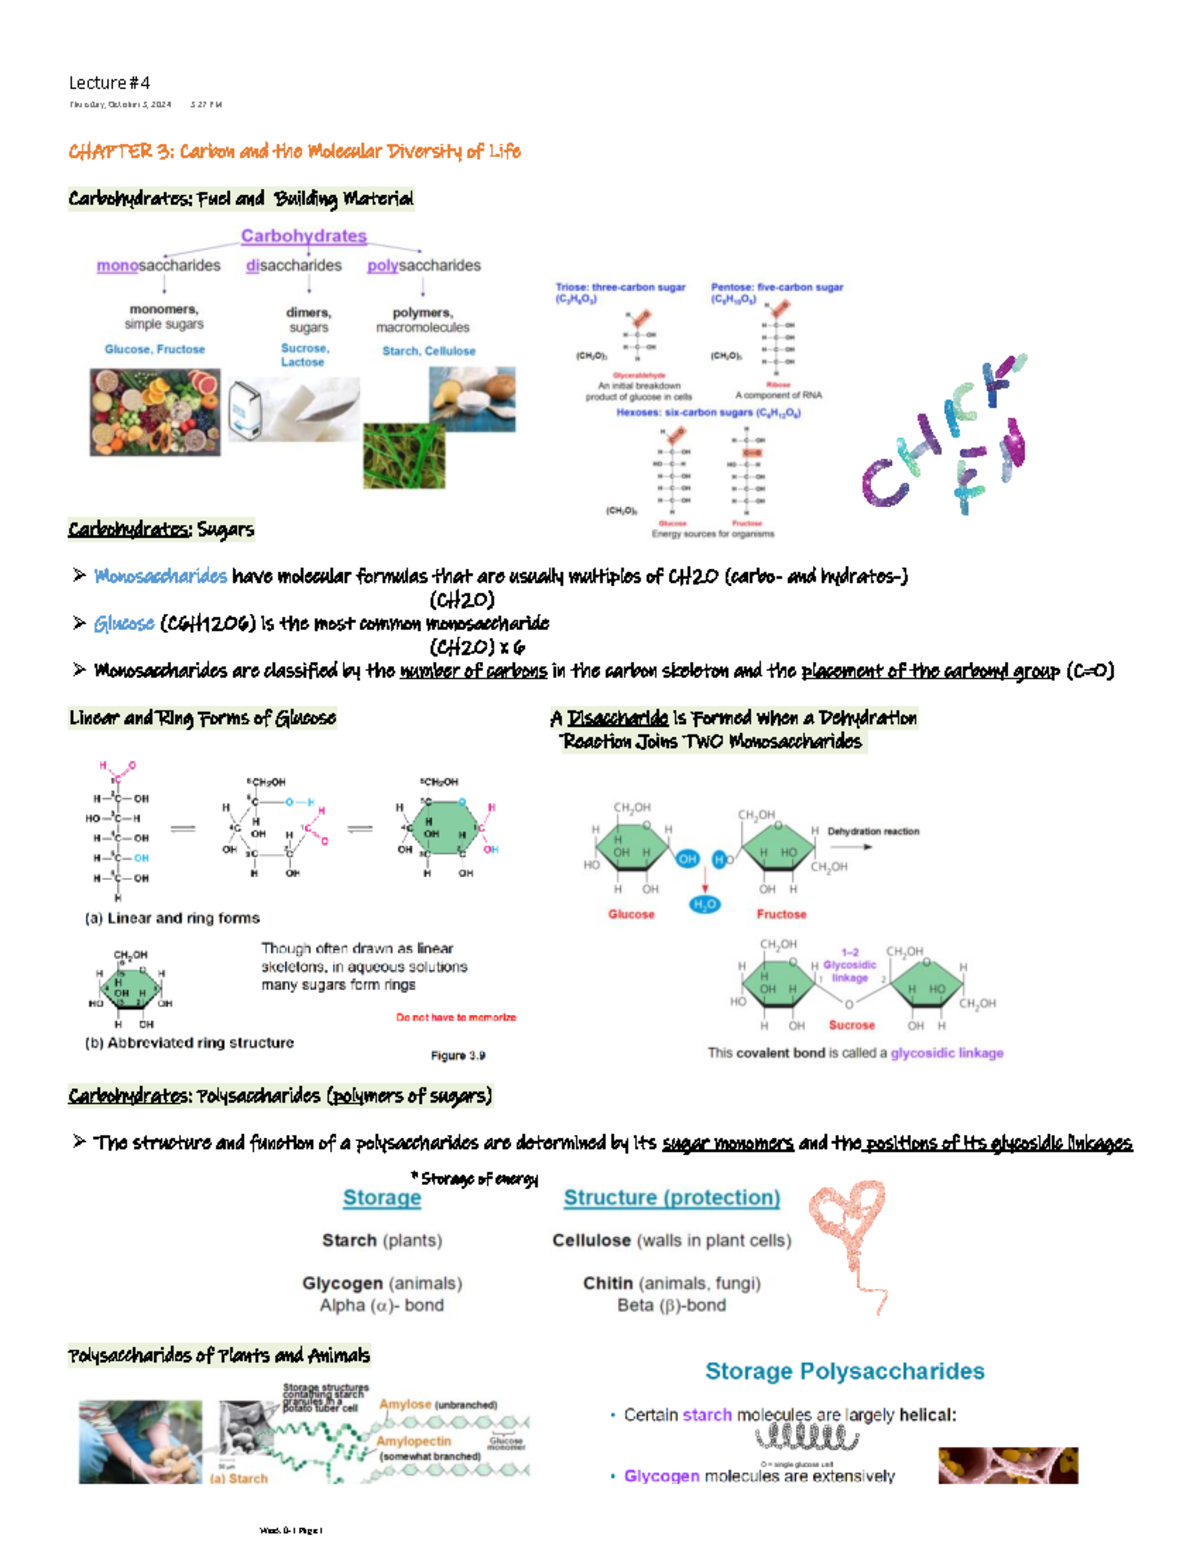
Carbohydrates, proteins, and nucleic acids are all polymers built from monomers. Lipids are the exception—they don't form true polymers in the same way. The bonds between monomers form through dehydration synthesis, which removes a water molecule. Breaking those bonds requires hydrolysis, which adds water back. The chemistry is simple. The bookkeeping is where students lose points on exams. A trisaccharide made from three glucose molecules contains two glycosidic bonds and releases two water molecules during formation. A polypeptide of 50 amino acids contains 49 peptide bonds and releases 49 water molecules. The pattern is consistent across all three polymer types. Recognize it early and you save time on calculation questions. Carbohydrate structure depends on linkage type. Alpha glycosidic bonds in starch create helical structures suited for energy storage. Beta glycosidic bonds in cellulose create straight, rigid chains suited for structural support. Humans digest starch because we produce amylase. We cannot digest cellulose because we lack cellulase. Herbivores solve this problem with symbiotic bacteria in their gut that produce cellulase. The difference between an alpha and beta bond is the orientation of a single hydroxyl group on the anomeric carbon. One bond orientation changes everything.
Get the Full Details
Proteins: Folding Is Where the Work Happens
Amino acids share a common structure: an amino group, a carboxyl group, a hydrogen atom, and a variable R group, all bonded to a central carbon. The R group determines the amino acid's properties. Twenty standard amino acids combine in essentially infinite sequences. The sequence determines the three-dimensional fold. Primary structure is the linear sequence. Secondary structure involves hydrogen bonding between backbone atoms, forming alpha helices and beta pleated sheets. Tertiary structure is the overall three-dimensional shape stabilized by interactions between R groups—hydrogen bonds, ionic bonds, disulfide bridges, and hydrophobic interactions. Quaternary structure involves multiple polypeptide chains assembling into a functional protein. Misfolding is the problem that kills cells. Prion diseases demonstrate this most dramatically. A misfolded protein template forces normally folded proteins into the same abnormal conformation. The aggregate damages neural tissue. This isn't theoretical. Creutzfeldt-Jakob disease and bovine spongiform encephalopathy follow this mechanism. The same principle applies to Alzheimer's and Parkinson's, though the specific misfolded proteins differ.
Nucleic Acids: Directionality Is Non-Negotiable
DNA and RNA are polymers of nucleotides. Each nucleotide contains a five-carbon sugar, a phosphate group, and a nitrogenous base. DNA uses deoxyribose. RNA uses ribose. DNA contains thymine. RNA contains uracil instead. The sugar-phosphate backbone creates directionality. One end has a free phosphate group—the 5' end. The other has a free hydroxyl group—the 3' end. All polymerization proceeds in the 5' to 3' direction. This directionality matters for replication, transcription, and every technique built on those processes. A common mistake is treating DNA and RNA as interchangeable. They share a backbone chemistry but differ in sugar, base composition, and typically in strand number. Double-stranded DNA is stable for long-term information storage. Single-stranded RNA is versatile but less stable. Cells use RNA for temporary tasks—messenger RNA, transfer RNA, ribosomal RNA. The structural difference between DNA and RNA explains why DNA is the archive and RNA is the working copy.
Where This Material Gets Tricky
The section on enantiomers is where most students hit a wall. The concept itself is straightforward—mirror-image molecules—but applying it to biological contexts requires understanding that enzymes are themselves chiral. An enzyme's active site has a specific three-dimensional shape. It binds one enantiomer and not the other. This isn't a minor detail. It determines drug efficacy and safety. The FDA requires enantiomeric purity testing for chiral drugs because the wrong enantiomer can be inactive, less effective, or harmful. Lipids are another friction point. The chapter groups them with the other macromolecules, but lipids don't polymerize. They assemble through hydrophobic interactions, not covalent bonds between repeating units. Triglycerides form from glycerol and three fatty acids through ester linkages. Phospholipids replace one fatty acid with a phosphate-containing group. The resulting amphipathic structure drives membrane formation spontaneously in aqueous environments. This self-assembly is energetically favorable and doesn't require enzymatic catalysis. That distinction matters for understanding how the first cellular boundaries could have formed.
Practical Study Approach
Draw the functional groups. Not from memory. Draw them from the textbook diagram, then redraw them from scratch. The act of drawing forces you to notice bond angles and atom connectivity. Flashcards work for the names and formulas, but they don't build the visual recognition you need for mechanism questions. Practice polymerization calculations until they become automatic. Given n monomers, how many bonds form? How many water molecules are released? The answer is n-1 for linear polymers. For branched polymers, the calculation changes. Know the difference. Focus on the relationships between structure and function. Cellulose is structural because of beta linkages. Starch is storage because of alpha linkages. The bond type determines the shape. The shape determines the function. This pattern repeats across every macromolecule class in the chapter. Once you see it, you stop memorizing and start reasoning.
The chapter title emphasizes molecular diversity. Carbon's four bonding capacity, combined with functional group chemistry and polymerization, produces the complexity that life requires. Understanding that mechanism—not just listing facts—carries you through the rest of the course.