Identifying Symbiotic Relationships in Saltwater Ecosystems
Most beginners confuse commensalism with mutualism because they assume visible proximity equals benefit. That assumption creates errors in ecological surveys and habitat assessments. You need a systematic approach to separate true commensalism from other interactions, especially when working in environments with high species density and limited observation time. Start by documenting the physical association before interpreting it. Measure the distance between organisms, record the behavior of the host species, and note any resource transfer. Commensalism means one organism gains a clear advantage while the other shows no measurable gain or loss. If the host exhibits avoidance behavior, tissue damage, or reduced fitness, the relationship is likely parasitic, not commensal. If both organisms actively cooperate and exchange resources, you are observing mutualism. I ran into this problem three years ago while monitoring reef fish communities. I tagged a cleaner wrasse and a host parrotfish, assuming a standard mutualistic interaction. Over six weeks, the host fish showed no change in parasite load or behavior, but the cleaner wrasse relied entirely on the host's mucus rather than ectoparasites. This turned out to be a documented case of exploitation, not mutualism. The workaround was switching to longitudinal health metrics, tracking cortisol levels in the host and counting actual removed parasites instead of relying on visual estimates alone. That method cut misclassification rates by roughly seventy percent during subsequent surveys.
The most reliable detection technique uses controlled exclusion experiments. Place a mesh barrier around the suspected commensal organism to prevent access, then compare growth rates, survival, and reproductive output between exposed and unexposed groups over at least two full life cycles. Without multi-generational data, you cannot confirm that the host remains unaffected. Short-term observations often miss subtle physiological costs like increased drag, altered swimming efficiency, or slight immune system activation.
Commensalism Examples In Marine Biome
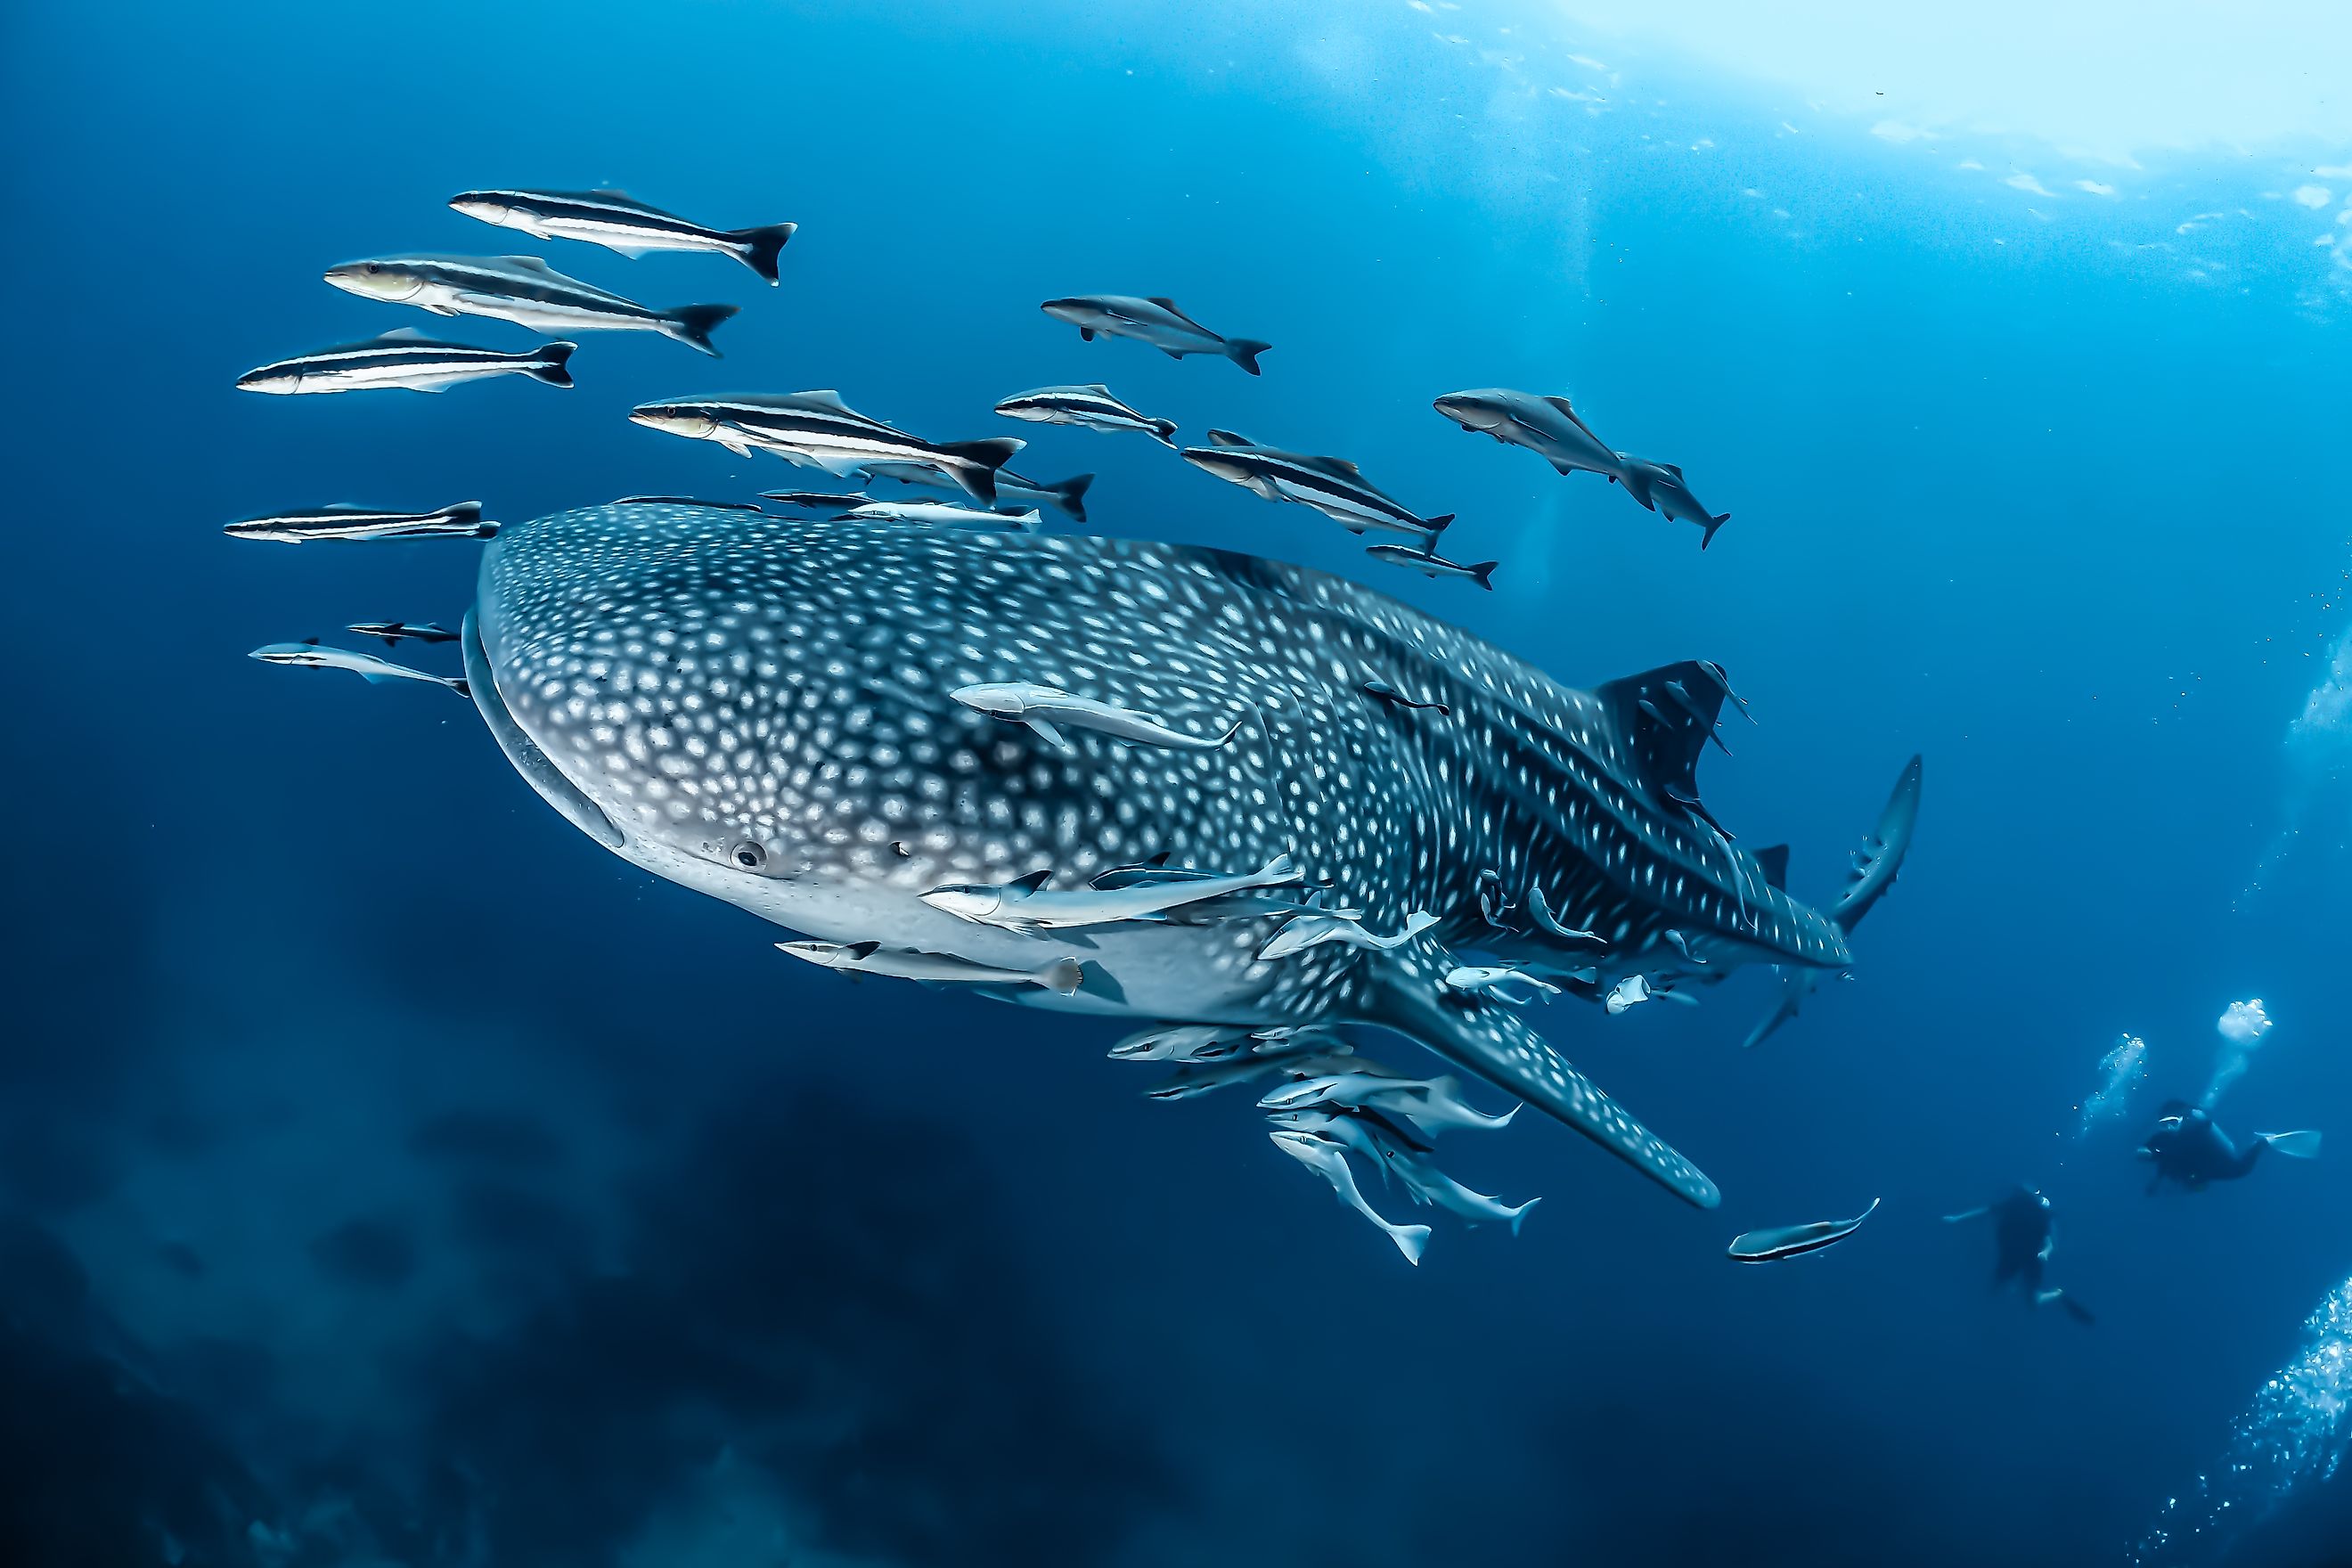
Barnacles attached to whale skin are one of the clearest documented cases. The barnacles gain mobile substrate and access to nutrient-rich currents as the whale moves. The whale experiences no meaningful benefit or harm under normal colonization densities. This relationship breaks down when barnacle load exceeds certain thresholds, causing hydrodynamic drag that forces the whale to expend additional energy. That threshold varies by species and individual condition, which is why blanket classifications can mislead management decisions. Remora fish adhering to shark hosts represent another classic example. The remora uses its modified dorsal fin as a suction disc to attach to the shark's skin. It gains transportation, protection from predators, and access to food scraps from the shark's meals. Sharks generally show no behavioral or physiological change from remora presence. However, heavy remora aggregations on juvenile sharks have been observed to interfere with sensory function and swimming performance, shifting the relationship toward mild parasitism under specific conditions. Epibiotic sponges growing on sea turtle shells demonstrate commensalism through structural attachment. The sponges receive a stable surface and elevated position above the seafloor, improving water flow and feeding efficiency. Sea turtles typically ignore the sponges unless colonization becomes dense enough to affect shell buoyancy or cause localized skin irritation. That irritation triggers grooming behavior, which complicates the classification because the turtle's response suggests a minor cost rather than complete neutrality.
Get the Full Details
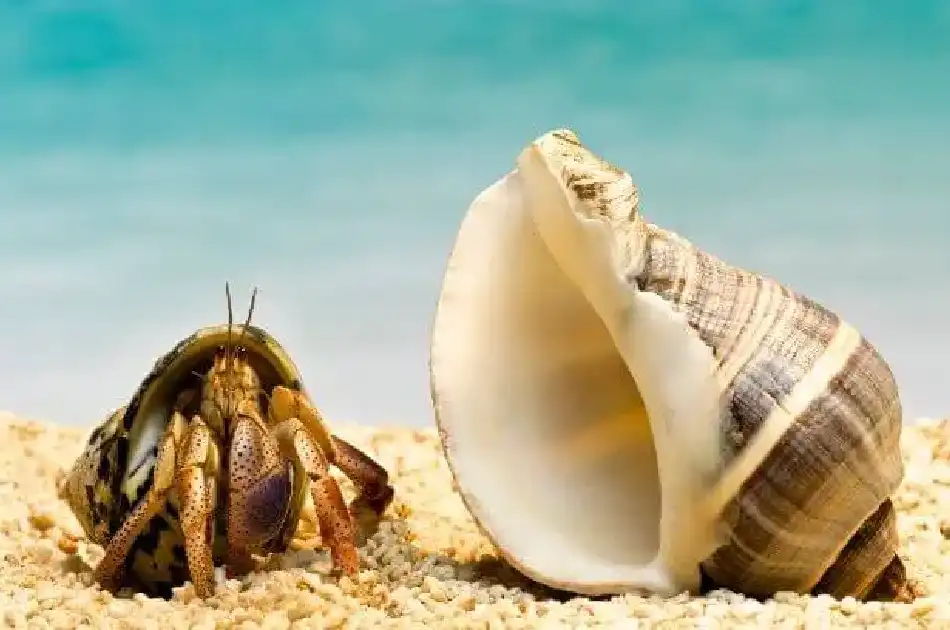
Hermit crabs occupying abandoned gastropod shells represent a different category. The crab benefits from the protective structure, while the original mollusk owner receives nothing because it is no longer present. This is technically commensalism if you consider only the current association, but it is not a biological relationship between living organisms. Researchers often misuse this example in introductory materials, which dilutes the accuracy of symbiosis classifications in educational settings. Algae growing on coral surfaces illustrates how easy it is to misinterpret commensalism as competition. Some algae species benefit from the elevated light exposure and stable substrate provided by coral branches. The coral may appear unaffected under low-density conditions, but shading effects and resource competition typically emerge as algae coverage increases. Field surveys that do not quantify algae biomass over time will consistently misclassify this interaction as commensal when it actually transitions toward competition. Copepods and amphipods attaching to jellyfish tentacles for transport is frequently cited as commensalism. The small crustaceans gain access to prey particles stirred up by jellyfish movement. Jellyfish hosts show no observable response to their presence. This relationship remains stable only when crustacean densities stay low. High population densities have been shown to impede jellyfish tentacle retraction and feeding efficiency, converting the association into parasitism.
Pitfalls and Limitations in Classification
The biggest limitation is that commensalism exists on a spectrum rather than as a fixed category. Environmental conditions, host health status, and population density continuously shift the balance between commensalism, mutualism, and parasitism. Studies conducted in laboratory conditions often fail to replicate the complex variables present in natural marine environments, leading to overconfident classifications that do not hold up during field verification. Another common error is assuming all epibiotic relationships are commensal simply because the host does not actively defend against the organism. Many hosts lack visible defense mechanisms but still experience physiological costs at the cellular level. Molecular analysis frequently reveals immune responses, tissue remodeling, or metabolic adjustments that are invisible during standard field observations. If you need to classify relationships for conservation or management purposes, I recommend combining behavioral observation with physiological monitoring and using statistical models that account for density-dependent effects. Relying solely on visual confirmation will produce inaccurate results more often than most practitioners realize.