Working With Bacterial Gene Transfer: A Practical Guide
Conjugation Transformation And Transduction
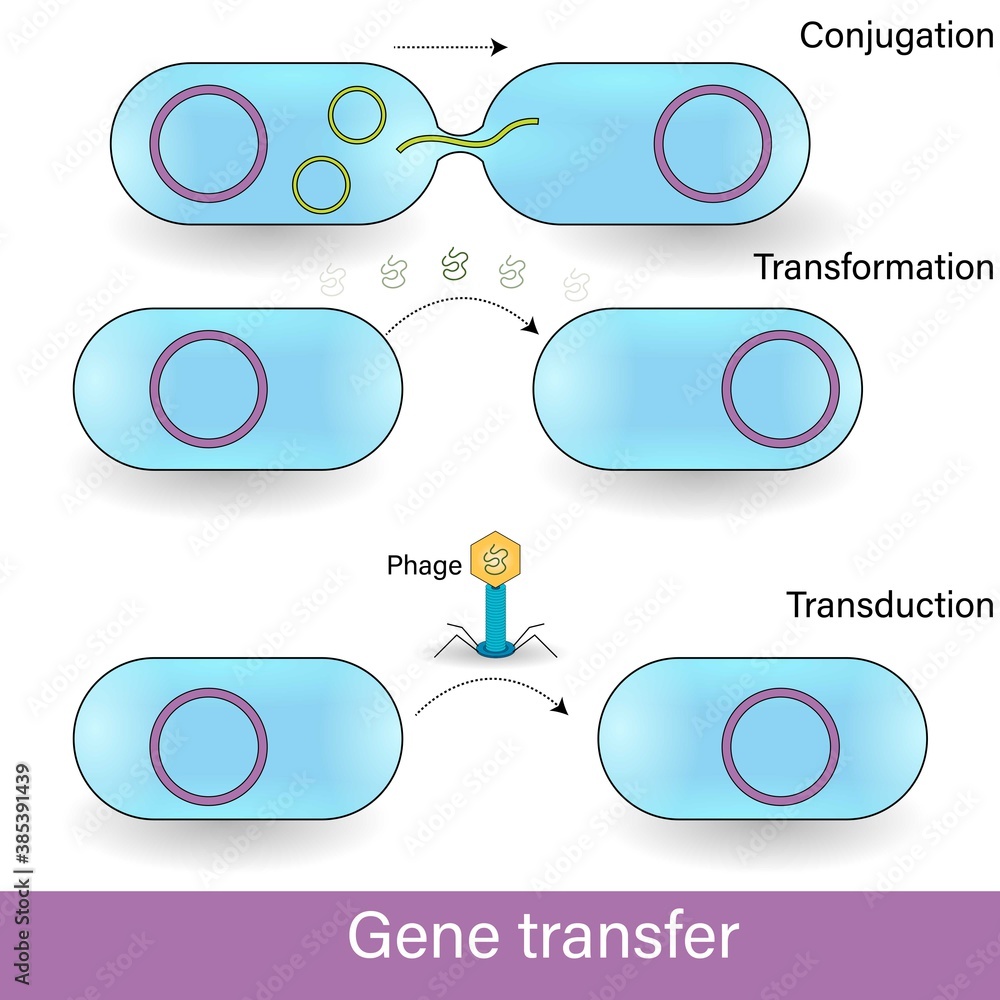
These three mechanisms are how bacteria move genetic material around. They come up constantly in cloning workflows, mutagenesis projects, and basic strain construction. Understanding the practical differences between them matters more than memorizing definitions. The failure modes are specific and painful if you skip the basics. Conjugation transfers DNA through direct cell-to-cell contact. A donor cell carries a conjugative plasmid or mobilizable element and builds a pilus to connect to a recipient. The DNA gets nicked at the origin of transfer and one strand moves across the mating bridge while the other is replicated in both cells. F-plasmids are the textbook example, but conjugative transposons and integrative conjugative elements are equally relevant in practice. The efficiency of this process depends heavily on growth conditions, cell density, and whether the recipient already carries incompatible plasmid families. If your donor and recipient share the same incompatibility group, the plasmid gets kicked out and your conjugation yield drops to near zero. I learned that one the hard way during a multi-plasmid strain construction project where two groups kept colliding. It cost me three weeks and a lot of wasted plates before I switched to compatible vectors. Transformation is the uptake of free DNA from the environment. In the lab, this usually means chemical competence with calcium chloride and heat shock, or electroporation for higher efficiency. The choice between methods matters more than people admit. Electroporation typically gives 10^8 to 10^9 transformants per microgram of supercoiled plasmid DNA with competent E. coli. Chemical transformation with standard protocols sits around 10^6 to 10^7 per microgram, though high-efficiency commercial prep kits can push that higher. The catch with electroporation is that salt concentration must be extremely low. Residual buffer salts from a miniprep elution will arc in the cuvette and destroy your cells. I once ran a full electroporation run with incompletely desalted DNA and got absolutely zero colonies. Spinning down and washing the DNA pellet three times in ice-cold water before elution solved it immediately.
Transduction moves DNA via bacteriophage. Generalized transduction packages random fragments of host DNA into phage capsids during the lytic cycle. Specialized transduction carries only DNA adjacent to a prophage integration site. P1 phage is the standard workhorse for generalized transduction in E. coli and related Enterobacteriaceae. P22 works for Salmonella. Mu phage handles both. The key advantage of transduction over plasmid-based methods is that it delivers DNA without requiring a selectable marker on the vector itself. You can move chromosomal markers cleanly. The limitation is host range. A phage that transduces one strain efficiently may not touch another, even within the same species. I hit this when trying to move a mutation between two closely related E. coli isolates using P1. The phage grew fine on the donor but produced zero transductants on the recipient. Switching to a broad-host-range conjugation system solved it, though it took longer overall. When you are planning an experiment, the first decision is what you are trying to move. Plasmids larger than 15 kilobases transfer poorly by transformation unless you use specialized high-efficiency protocols. Conjugation handles large constructs better, especially broad-host-range plasmids like RSF1010 derivatives. Transduction struggles with anything larger than the phage packaging limit, which is roughly 2 to 4 kilobases depending on the system. This size constraint is a hard limit, not a soft recommendation. Marker rescue is another practical consideration that trips people up. After conjugation or transduction, you need to select for the transferred DNA without losing other markers you want to keep. Counter-selection with sacB or rpsL works well for chromosomal swaps but introduces extra steps. For simple plasmid transfers, antibiotic selection on the donor plasmid is sufficient. The problem arises when the recipient already carries resistance to the same antibiotic. Always check the resistance profiles of both strains before picking your selection markers. A quick PCR screen of your recipient strain for common resistance genes can save you from redesigning the whole construct later.
The timeline for each method varies significantly. Chemical transformation takes about 45 minutes of active work plus overnight growth. Electroporation is faster, maybe 20 minutes active time. Conjugation requires a mating step of 1 to 4 hours, then plating and selection, so expect results in 18 to 24 hours. Transduction involves growing the phage lysate first, which takes another 12 to 16 hours before you even start the transduction itself. If you need results quickly, transformation is your best bet. If you are moving large constructs or working across species, conjugation is the more reliable path despite the longer timeline. One thing people overlook is the role of restriction-modification systems in limiting the success of all three methods. A recipient strain with active restriction enzymes will chop up incoming foreign DNA before it can establish itself. This is why many lab strains carry modifications like dam/dcm deficiencies or come from restriction-deficient backgrounds. When working with environmental isolates or less common species, restriction barriers can reduce transformation and transduction efficiency by orders of magnitude. In those cases, methylation of the incoming DNA to match the recipient pattern, or using a dam+/dcm+ donor strain, can dramatically improve outcomes. I encountered this when transforming plasmid DNA prepared from a dam+ strain into a restriction-sensitive K-12 derivative. The transformation efficiency was roughly one percent of what I expected. Methylating the DNA in vitro with the appropriate methyltransferases restored normal efficiency. If you need to move genetic material between distantly related species where conjugation and transduction both fail, nucleofection or protoplast transformation are fallback options. These are less efficient and more technically demanding, but they bypass the host-range constraints entirely. Protocols exist for many Gram-negative and Gram-positive species, though success is never guaranteed. The key is having a well-prepared competent cell suspension and fresh, high-quality DNA. Degraded DNA destroys any chance of recovery regardless of the method you use.
Get the Full Details


