Cellular Respiration Is Just Controlled Burning
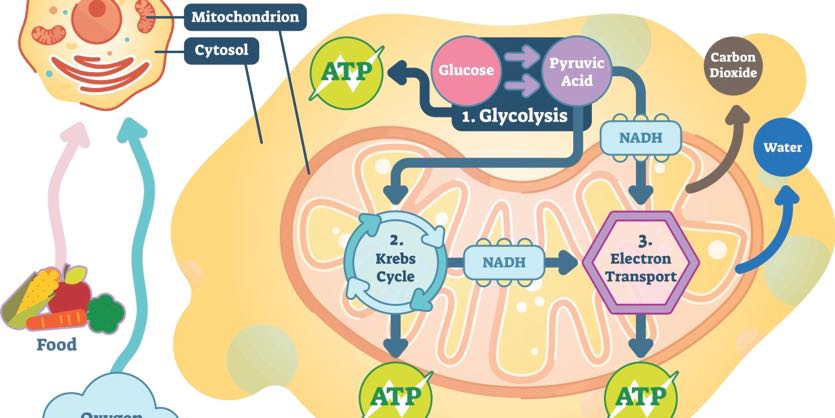
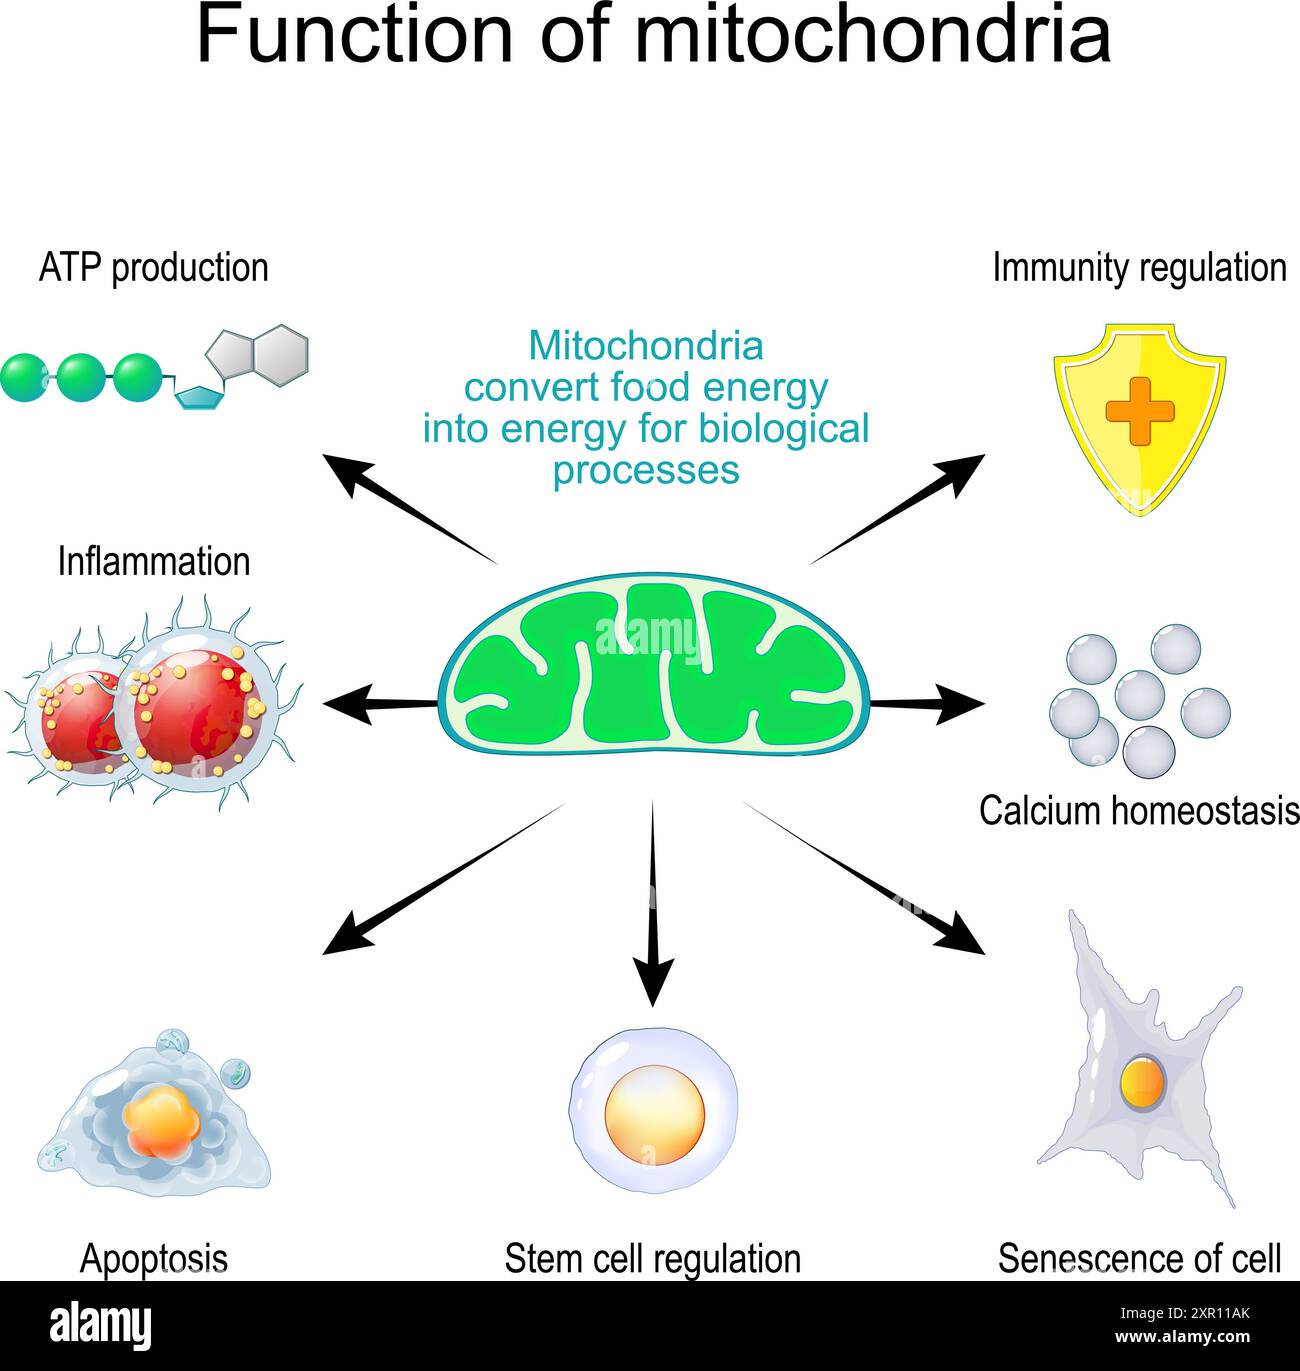
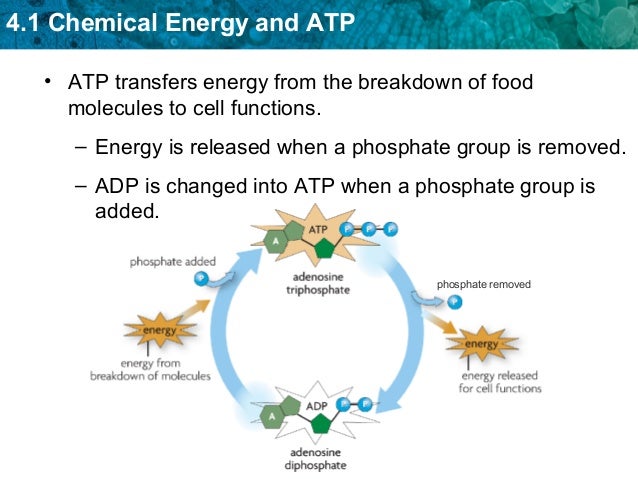
You take in glucose or fatty acids. Your mitochondria break them down in a series of steps that release energy, which gets captured in ATP. That is essentially what Converts Food Into Atp For The Cell. It is not magic. It is chemistry happening at 37 degrees Celsius inside a membrane-bound organelle. It starts in the cytoplasm with glycolysis, which splits one glucose molecule into two pyruvate molecules and nets you two ATP and two NADH. That part is straightforward and does not even require oxygen. From there, pyruvate enters the mitochondrion, gets converted to acetyl-CoA, and enters the Krebs cycle. The Krebs cycle produces more NADH, some FADH2, and a small amount of GTP, which your cell can use directly as ATP. All of those electron carriers then feed into the electron transport chain embedded in the inner mitochondrial membrane. The electron transport chain is where the real work happens. Electrons move through complexes I through IV, and the energy released pumps protons from the matrix into the intermembrane space. This creates an electrochemical gradient. Protons want to flow back into the matrix, but the membrane is impermeable to them except through ATP synthase. As protons flow through that rotor, it spins and synthesizes ATP from ADP and inorganic phosphate. Oxidative phosphorylation typically yields around 26 to 28 ATP per glucose molecule, bringing the total yield to roughly 30 to 32 ATP.
Fatty acids enter through beta-oxidation, which chops them into two-carbon acetyl-CoA units. Each round of beta-oxidation also produces NADH and FADH2. A single palmitate molecule, for instance, generates significantly more ATP than a single glucose molecule. That is why fats are denser energy storage. But the cell cannot switch between fuel sources instantly. There is regulation, and the enzymes have preferences.
The Common Misunderstandings
Most people think ATP is some kind of universal free energy that you can just summon at will. It is not. ATP is a currency, and the cell has to earn it. The conversion process is tightly coupled to the proton gradient. If the membrane becomes leaky, everything slows down. Uncoupling proteins exist for a reason, but they burn substrate without making ATP. Brown fat uses this on purpose for thermogenesis in infants and hibernating mammals. In adult humans, it is less active, but it is still there. Another thing beginners miss is that glycolysis and the Krebs cycle are not just linear pathways. They are nodes in a much larger metabolic network. Intermediates get siphoned off for amino acid synthesis, for heme production, for gluconeogenesis when you are starving. The cell is constantly rebalancing. ATP demand from one tissue does not automatically mean another tissue shuts down its production. Different cell types run different metabolic programs depending on their function.
Get the Full Details
What Happens When It Breaks Down
I spent time troubleshooting a lab culture where cell metabolism was dropping faster than expected, and I kept chasing the wrong variable at first. I assumed it was a reagent issue or contamination. What I actually found was that the initial plating density was too high. At high confluency, cells shift from oxidative phosphorylation to aerobic glycolysis, the Warburg effect, even when oxygen is plentiful. They start producing lactate, the pH of the medium drops, and ATP output per glucose molecule decreases dramatically because glycolysis only yields two ATP compared to thirty-something from oxidative phosphorylation. The fix was simply re-plating at a lower density and allowing the cells to metabolize through respiration before any downstream assay. It sounds obvious now, but I wasted about two weeks on it before catching it. This kind of issue comes up repeatedly if you are measuring metabolic rates in any experimental setup. Oxygen consumption rate and extracellular acidification rate are the standard readouts, but you need to make sure the conditions actually support mitochondrial function. Damaged mitochondria, depleted cofactors like magnesium or B vitamins, or even suboptimal temperatures can all throttle ATP production. There is no single point of failure because the system is redundant by design.
What Converts Food Into Atp For The Cell in Practice
In practice, understanding this pathway matters whenever you are dealing with anything that involves cellular energy. This includes exercise physiology, where muscle fibers switch between fast glycolytic and slow oxidative fibers depending on intensity. It matters in disease states like mitochondrial myopathies, where mutations in mitochondrial DNA impair the electron transport chain. It matters in cancer research, where the metabolic reprogramming I mentioned above is a hallmark. And it matters if you are just trying to understand why eating a fatty meal keeps you satiated longer than a carbohydrate-heavy one. The key insight most people miss is that ATP is not the end product. It is the intermediate. The actual goal of metabolism is to maintain homeostasis, and ATP is just how the cell pays for it. When ATP levels drop, AMPK activates and signals the cell to increase fuel uptake and oxidation. When ATP is abundant, mTOR signals growth and biosynthesis. The whole system is a feedback loop, not a one-way street.
Limitations and When the System Fails
The mitochondrial ATP production pathway has real bottlenecks. One is oxygen availability. The electron transport chain stops working without an acceptor for those electrons at complex IV. Hypoxia shuts down oxidative phosphorylation entirely, and the cell falls back on anaerobic glycolysis, which is far less efficient and produces lactate as a byproduct. Lactate accumulation is what causes that burning sensation in muscles during intense exercise, and it also depresses cellular function if it gets too high. Another limitation is mitochondrial DNA damage. Unlike nuclear DNA, mtDNA lacks robust repair mechanisms and sits right next to the electron transport chain, which leaks reactive oxygen species as a natural byproduct. Over time, this causes cumulative damage. Some theories of aging tie directly to this. The body can mitigate it through mitophagy, the selective degradation of damaged mitochondria, but that process also declines with age. If you are looking for a way to enhance ATP production beyond what normal physiology allows, the evidence is mixed. Supplements like CoQ10 and D-ribose are widely sold, but their effectiveness depends entirely on whether you have a deficiency or a specific pathological condition. In healthy individuals with normal mitochondrial function, extra CoQ10 does not meaningfully increase ATP output. The system self-regulates. If you want to improve mitochondrial density and efficiency, exercise remains the only intervention with consistent, reproducible evidence behind it. Even then, the improvements are modest and take months to develop.