Atoms Are the Smallest Units That Still Matter in Living Systems
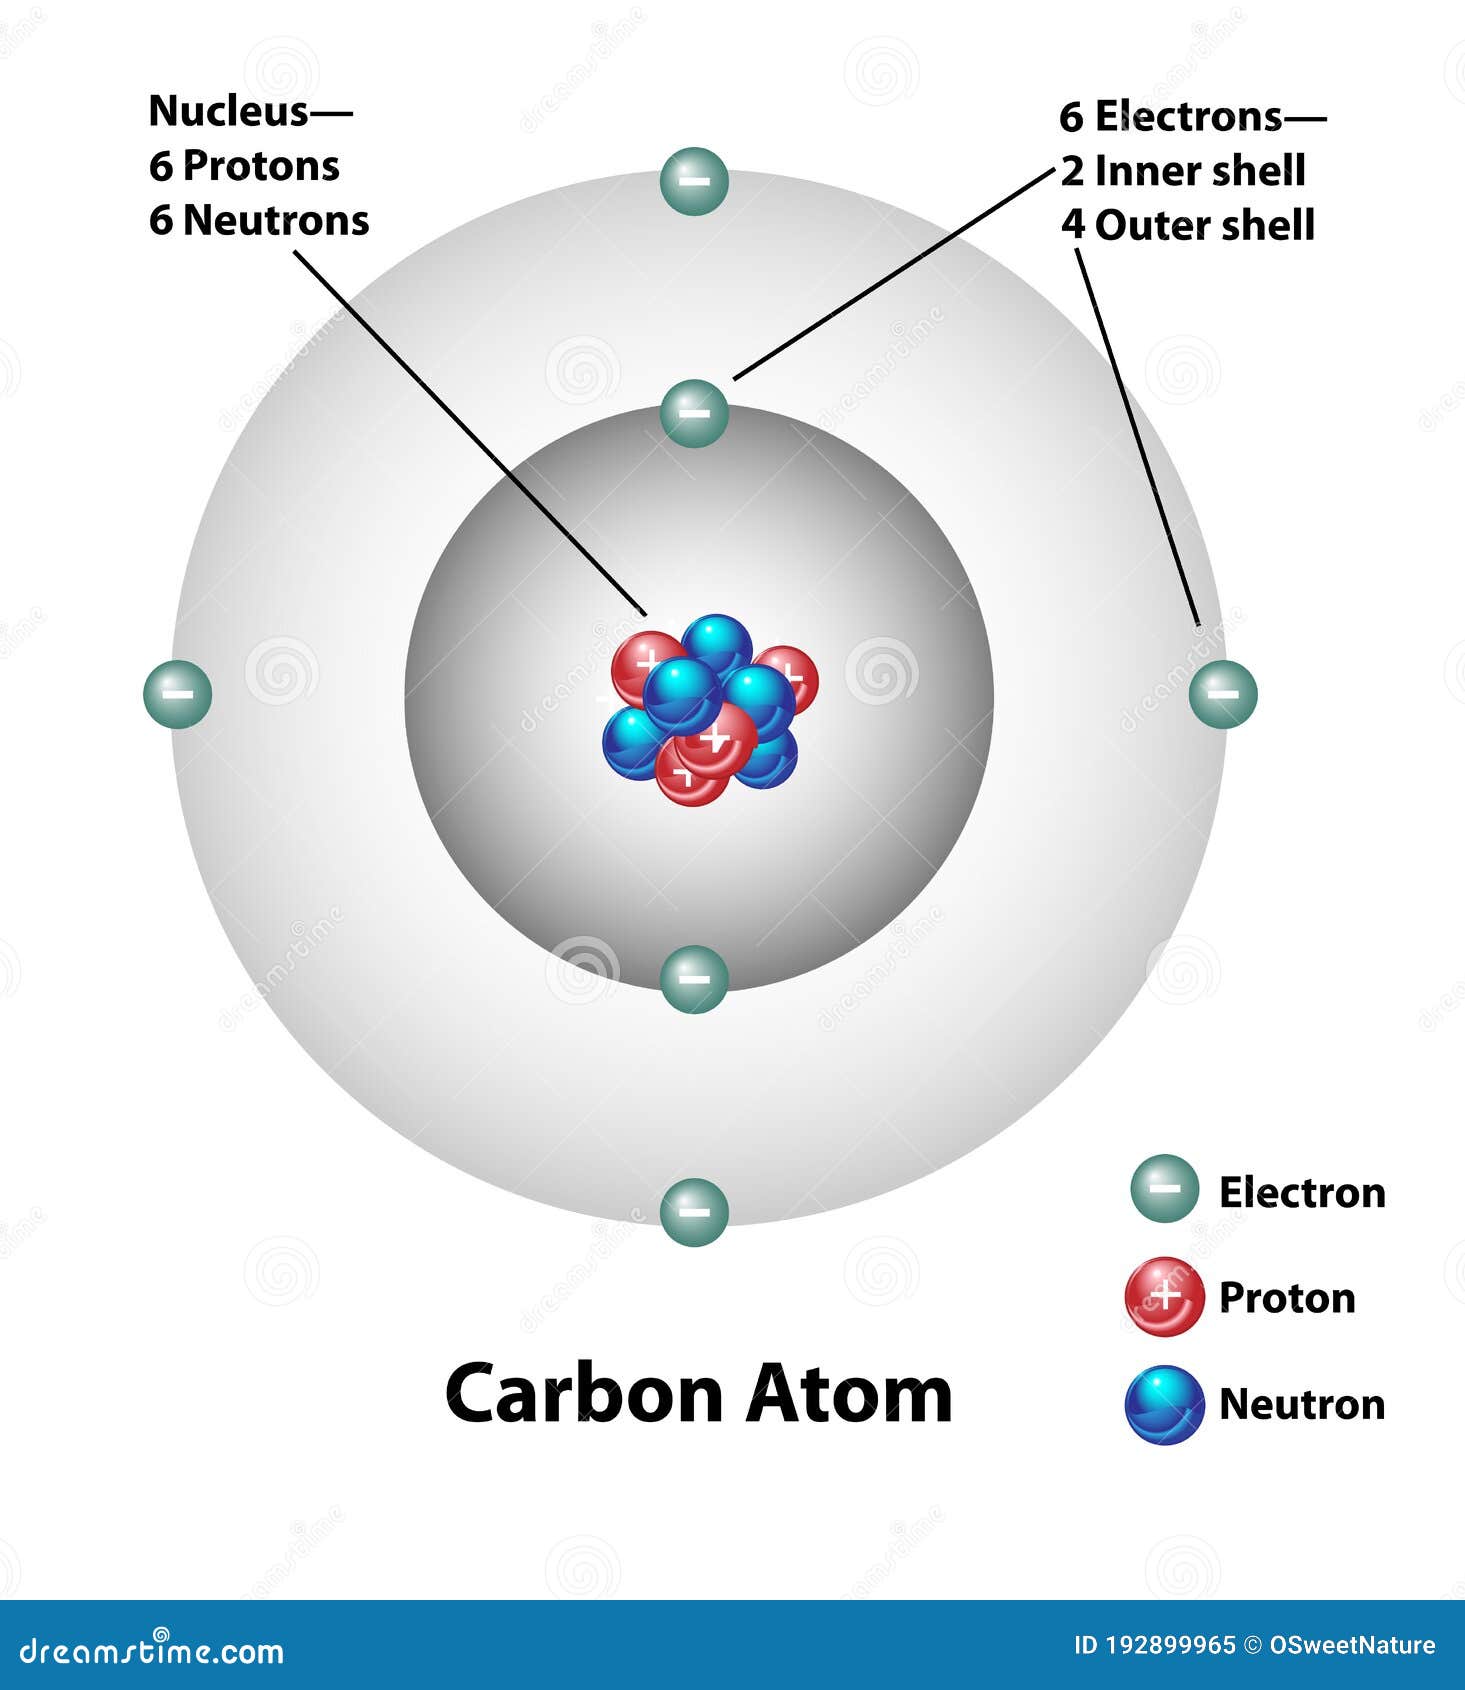
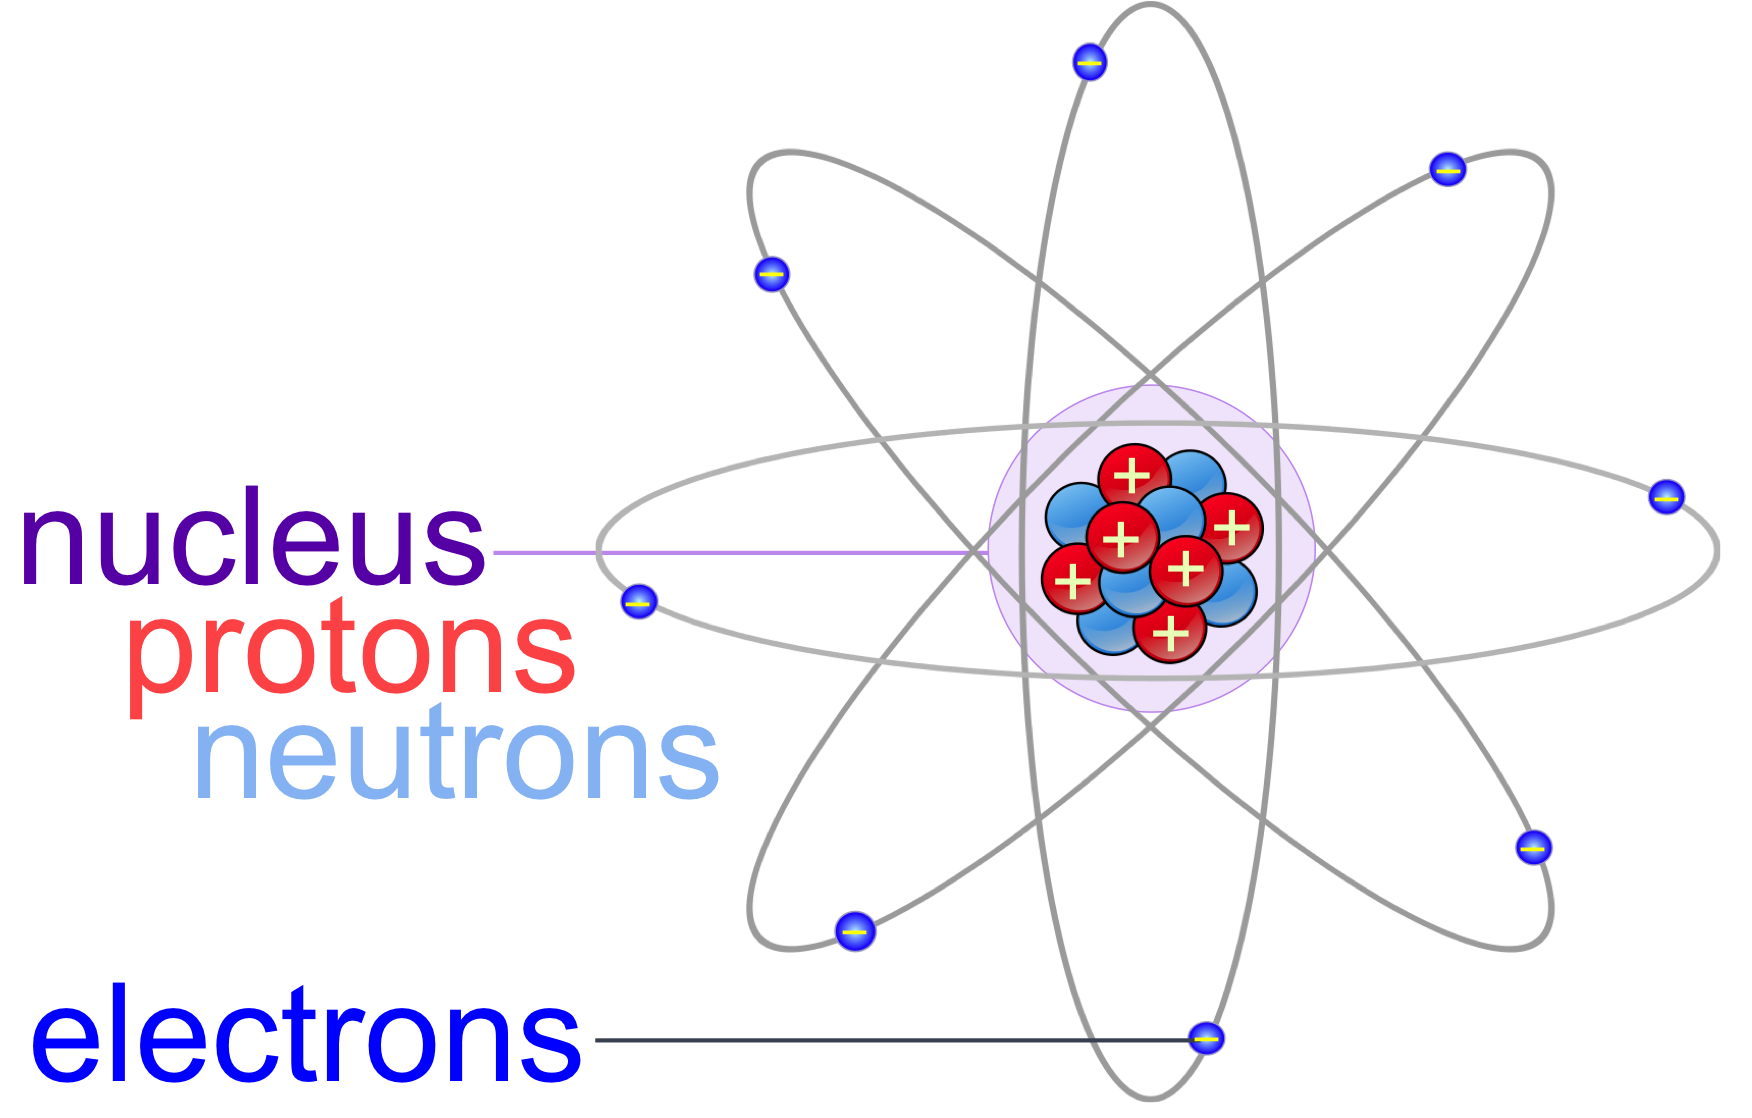
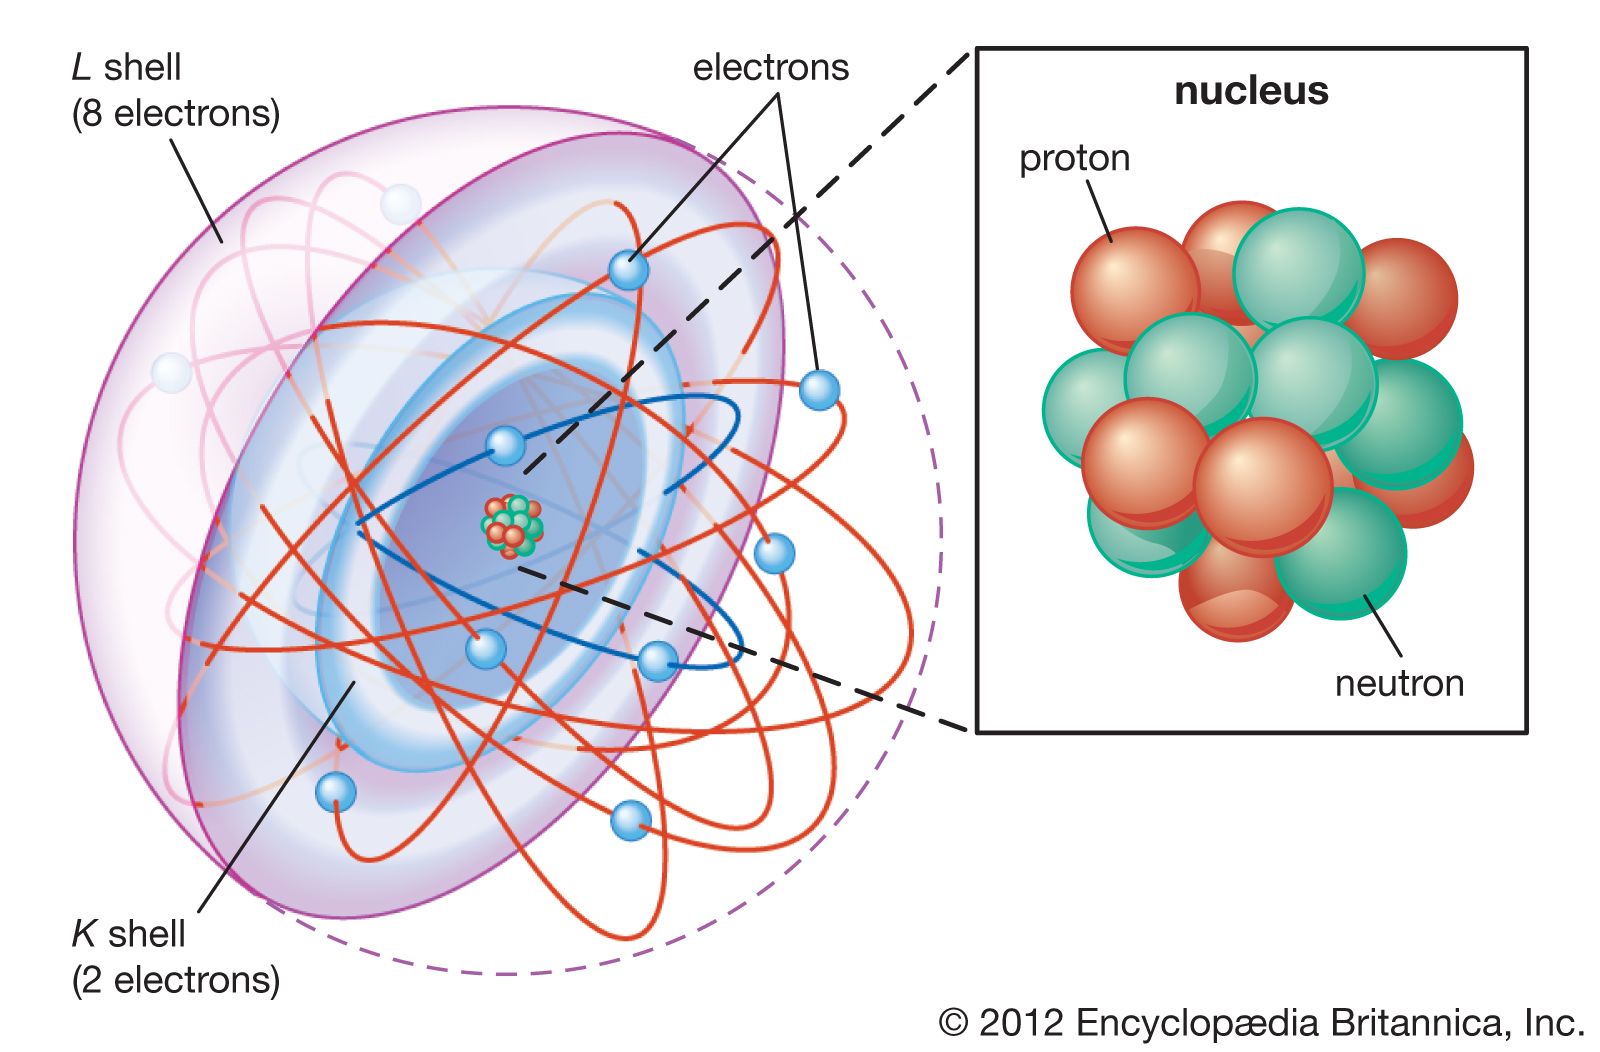
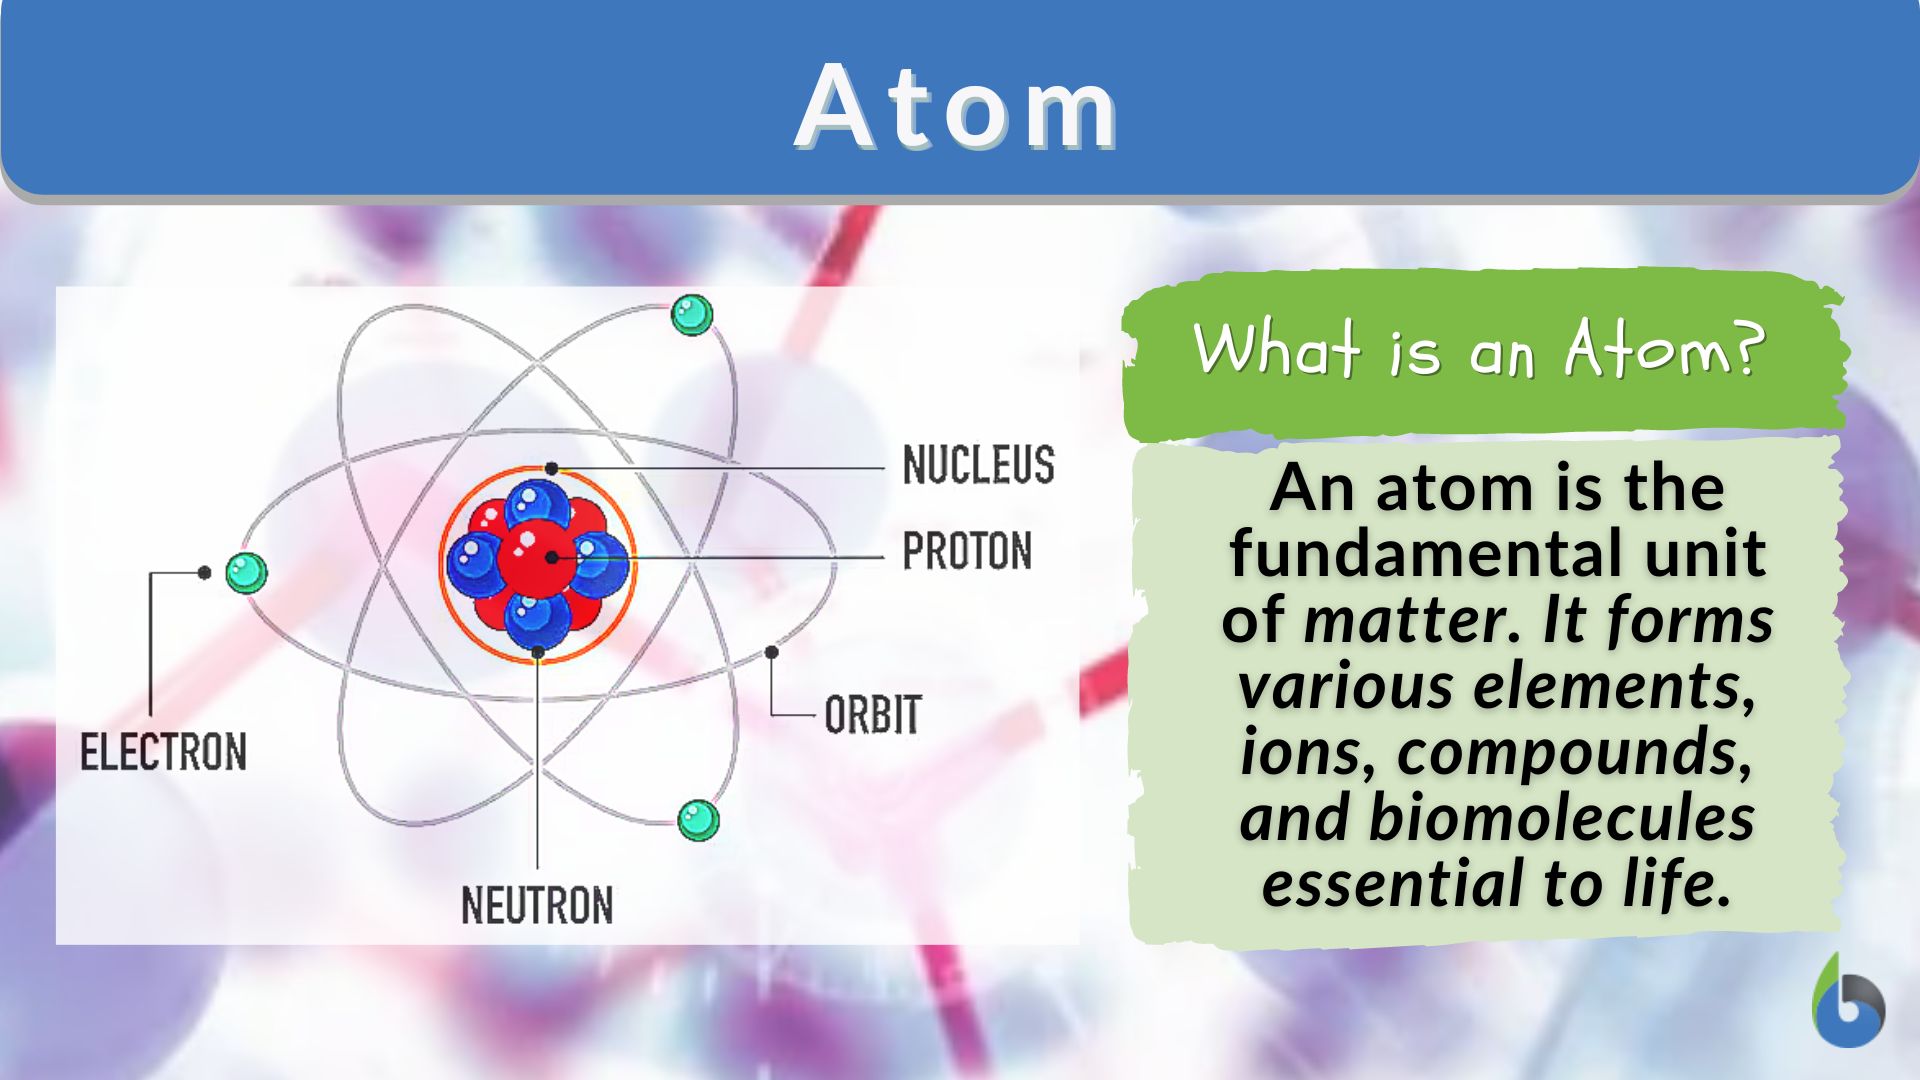
You open any biology textbook and somewhere near the beginning you get the periodic table dressed up as a prerequisite. This isn't filler content either. The reason carbon, hydrogen, nitrogen, oxygen, phosphorus, and sulfur show up repeatedly in metabolic pathways isn't because a curriculum designer likes memorization drills. It's because these six elements form roughly 96 percent of the dry mass of any organism you can identify on a phylogenetic tree, and the chemistry they support is non-negotiable. When I talk about how to define atom in biology, I usually start by pointing out that biology doesn't really have its own atomic theory. It borrows the physics and chemistry version wholesale and then asks what happens when you pile those atoms into structures that self-replicate, maintain ion gradients, and occasionally catch on fire if you heat them enough. The definition shifts depending on which layer you're standing at. At the molecular level an atom is a nucleus surrounded by electron orbitals and nothing more interesting than that. At the cellular level it becomes a participant in electrochemical gradients that power ATP synthase. At the organismal level it can be a diagnostic tracer in a PET scan or a toxic contaminant that accumulates in adipose tissue over forty years.
What You Actually Need to Define Atom In Biology Without Wasting Time
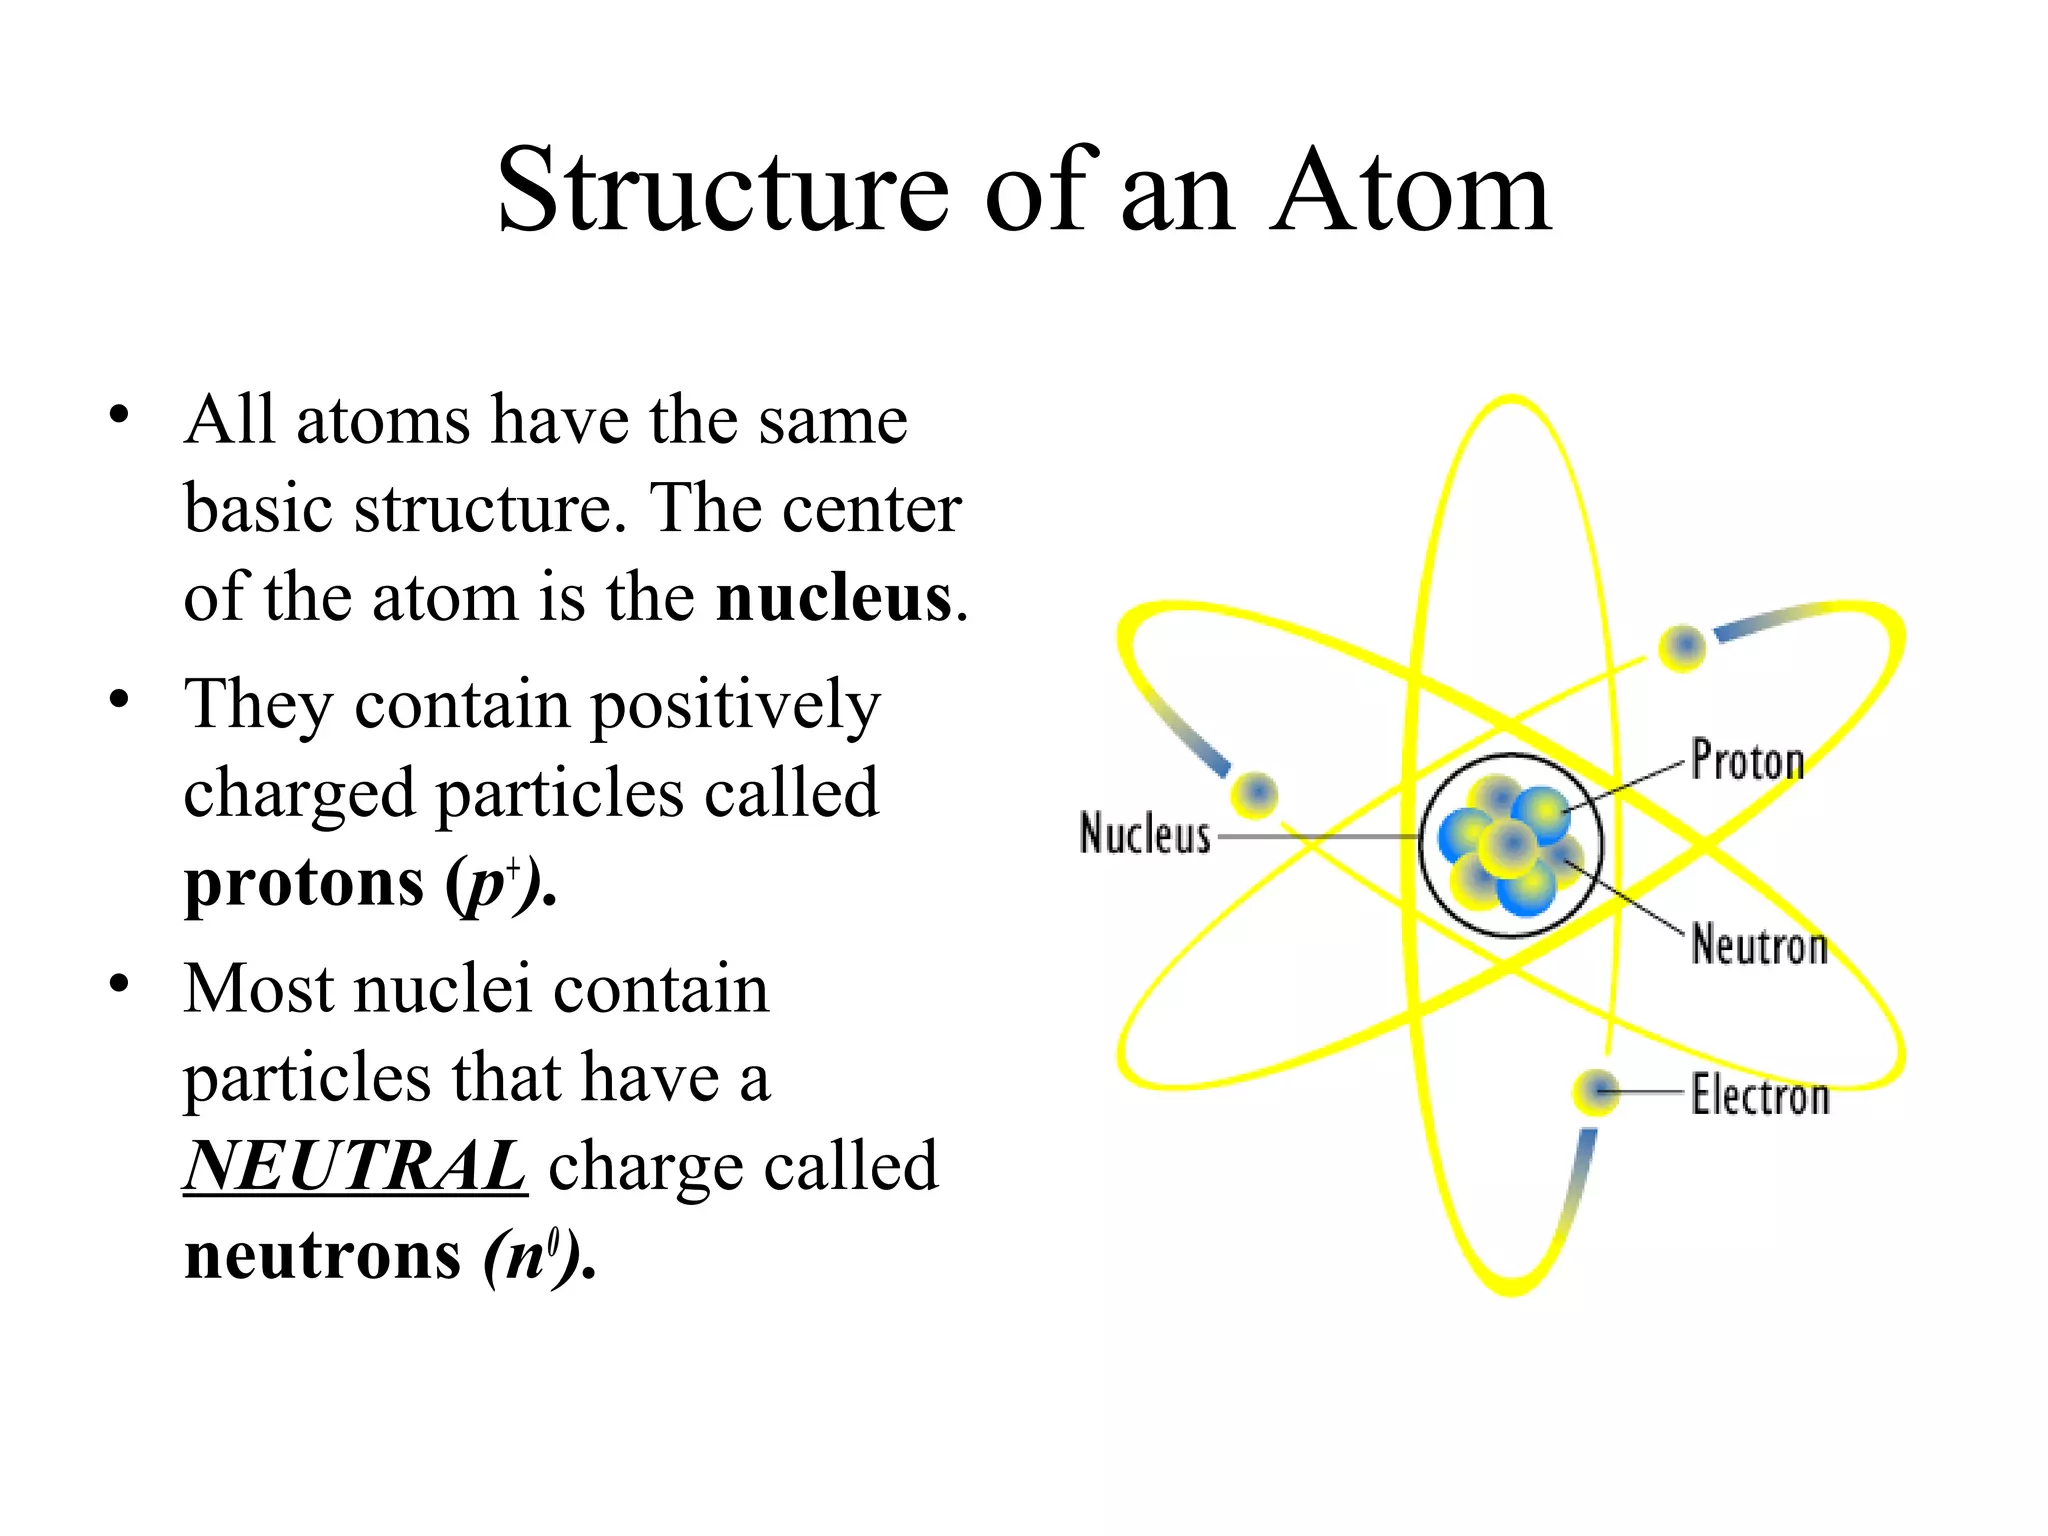
The definition that works in practice is short. An atom in biology is the smallest identifiable unit of an element that retains the chemical properties necessary to form the bonds and structures underlying cellular function. Anything smaller, like a bare nucleus or an isolated electron, stops participating in biochemistry and starts behaving like radiation or plasma instead. I once spent three weeks debugging why a stable isotope labeling experiment in cultured primary hepatocytes kept showing nonspecific scattering in the mass spectrometry readout. The issue was not the spectrometer. It was that I had defined my atom of interest too loosely. I was tracking carbon-13 enrichment in glucose but forgot that the cells were also pulling environmental CO2 through carbonic anhydrase activity, which scrambled the isotopic signature in the bicarbonate pool. Once I sealed the culture headspace and switched to measuring lactate enrichment instead of free glucose, the data became clean. The lesson was boring but useful: in biology you have to define which atom, in which molecule, in which compartment, before you can trust any number that comes out of an instrument. Most beginners treat atoms like interchangeable Lego bricks. They are not. Isotopes matter in ways that are easy to overlook until a protocol fails. Deuterium substitution changes bond vibration frequencies and can slow enzymatic turnover by a measurable amount. That is the kinetic isotope effect, and it is why some metabolism studies deliberately use deuterated substrates to map rate-limiting steps. If your lab uses normal light water and you switch to D2O without recalibrating osmolarity and enzyme kinetics, you will confuse an artifact with a biological finding. That happened to me with a cell line that stopped dividing after I accidentally prepared media in deuterated buffer. The cells were fine once I corrected for it, but the first forty-eight hours looked like a drug effect and wasted a lot of sequencing budget.
Another thing people miss is that the definition changes when you cross into metal biology. Iron in hemoglobin is not just an atom. It is a coordinated center inside a porphyrin ring, held in a specific oxidation state by histidine ligands, and its redox potential is tuned by the protein environment. Remove the protein and Fe2+ oxidizes to Fe3+ and precipitates as ferric hydroxide in minutes at physiological pH. The atom itself did not change identity. The system around it did. That is why bioinorganic chemistry exists as a subfield instead of being an aside in general biology. If you want a definition that holds up under peer review, include the compartment. An atom floating in cytoplasm is chemically distinct from the same atom buried in a membrane bilayer, which is distinct from the same atom sequestered in a lysosome at pH 4.8. The local dielectric constant, proton concentration, and coordination chemistry rewrite the reactivity of every element on the periodic table in predictable ways. That is not philosophy. It is why chelation therapy works for lead poisoning and why free copper kills cells through Fenton chemistry. The downsides of treating atoms as simple building blocks are real and they show up in grant reviews. If your mechanistic model says an enzyme works by positioning a catalytic residue near a substrate, reviewers will ask whether you checked the pKa shift caused by the local electrostatic field. They are right to ask. The atom is not just sitting there. The protein environment moves its electron density, changes its protonation state, and sometimes turns a weak nucleophile into a strong one. Ignoring that makes your model wrong in a way that is cheap to catch if you run a simple pH dependence assay and expensive to catch if you publish first.
Get the Full Details
I usually recommend starting with the six-element framework and then expanding only when the question demands it. Calcium signaling, magnesium-dependent phosphorylation, zinc finger domains, selenium in glutathione peroxidase, iodine in thyroid hormone. Each addition changes how you model the system. Each addition is worth learning because each one explains a disease mechanism or a drug target that the base six do not cover. Potassium channels, for instance, are not interesting because potassium is special. They are interesting because the selectivity filter uses a precise arrangement of carbonyl oxygens that mimics potassium's hydration shell well enough to strip water molecules without paying an energy penalty. That is atomic-scale design that looks like magic until you draw the crystal structure. For most people who need a working definition, this is sufficient. An atom in biology is the smallest unit of an element that participates in biomolecular structure or reactivity within a defined cellular compartment, with properties shaped by its chemical environment rather than by the atom alone. Everything else is detail you add when the experiment forces you to care about it.