Understanding How Cells Actually Use Energy
I spent about three years grading introductory biology papers before I stopped trying to rewrite the same misconceptions over and over. The ATP definition shows up in almost every exam, and almost every student gets at least part of it wrong. Not because the material is hard, but because the way it is taught skips the actual mechanism and lands on a memorization trap. Adenosine triphosphate is a nucleotide derivative composed of adenine, a ribose sugar, and three phosphate groups linked in series. The bonds between those phosphates are what matter. Specifically, the two terminal phosphoanhydride bonds store significant free energy not because the bonds themselves are especially strong, but because the products after hydrolysis are substantially more stable than the reactants. That is the part most textbooks gloss over.
What the Definition Of Atp Biology Actually Means
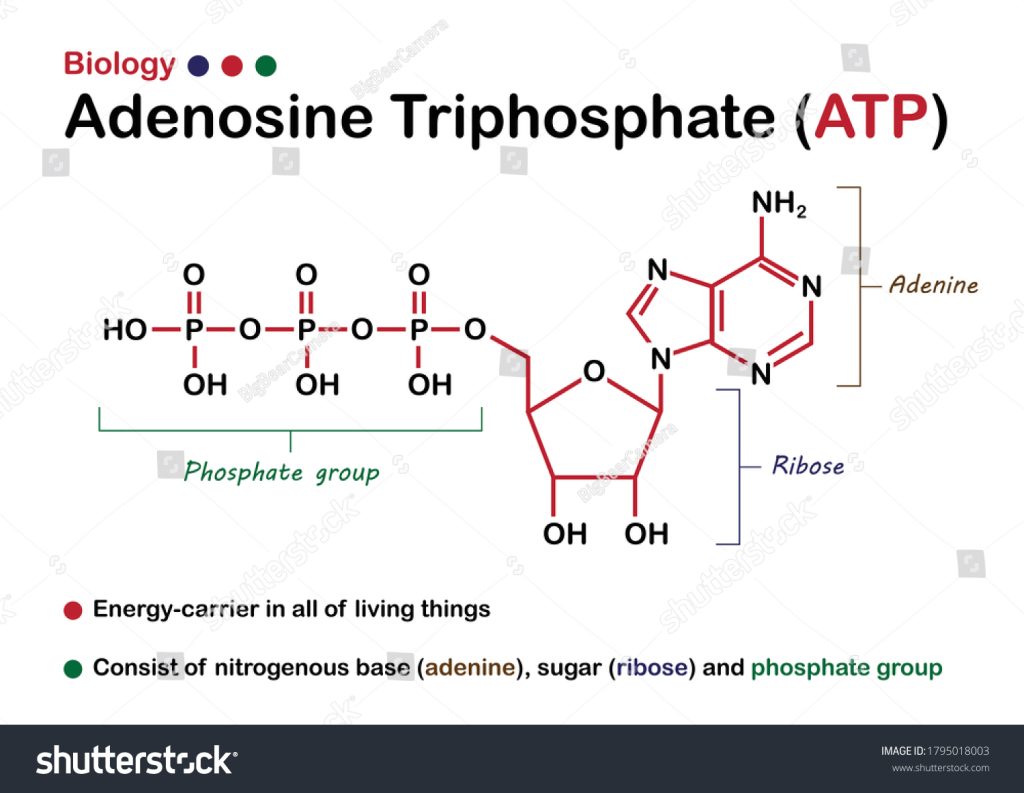
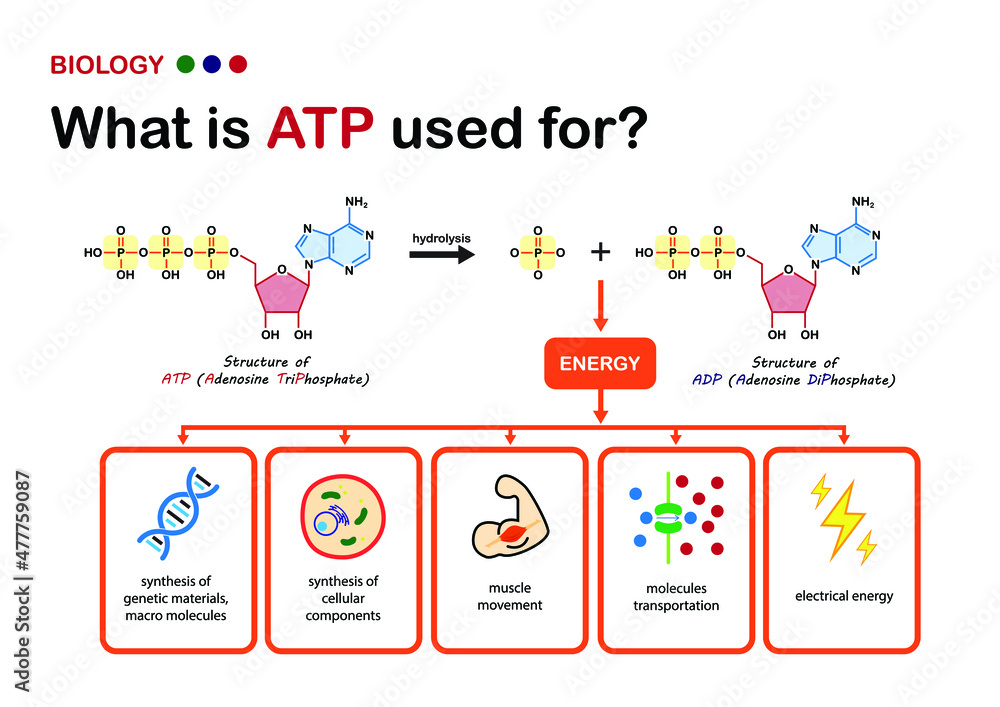
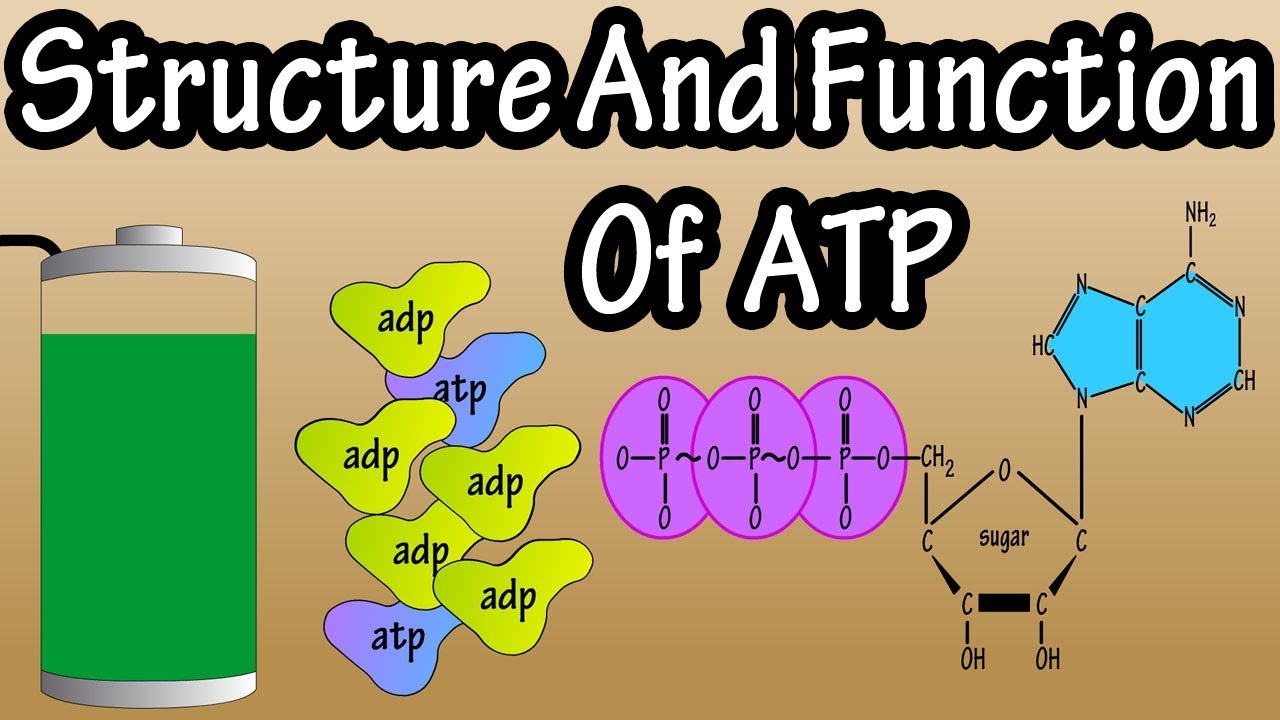
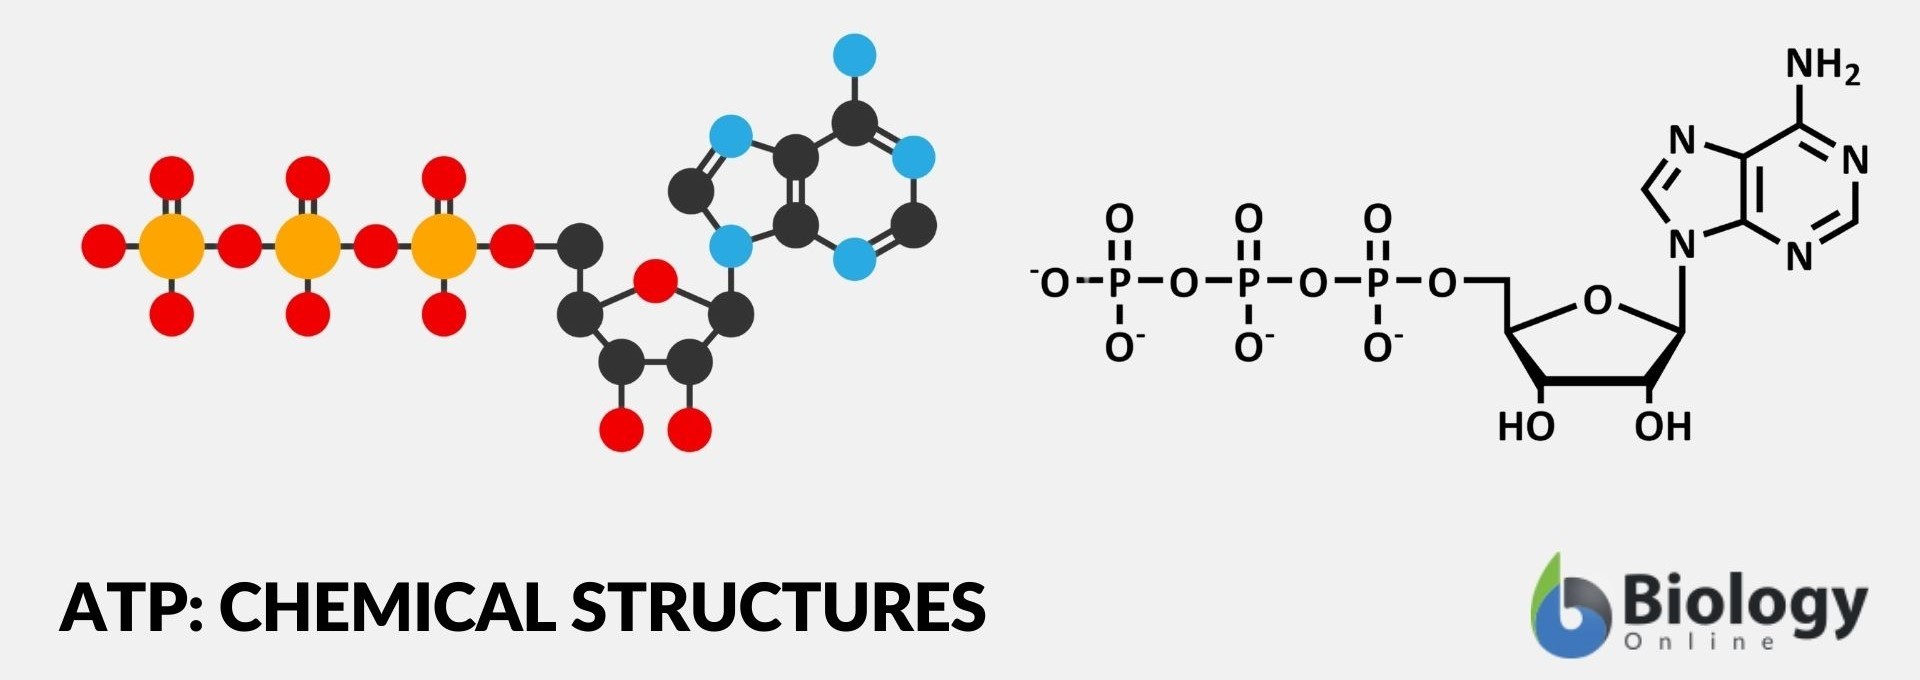
The standard definition will tell you ATP is the primary energy currency of the cell. That is technically correct and practically useless without context. A better framing: ATP couples exergonic and endergonic reactions through shared intermediate steps. When ATP hydrolyzes to ADP and inorganic phosphate, the released energy drives processes that would not occur spontaneously on their own. Protein synthesis, active transport across membranes, muscle contraction, and signal transduction all depend on this coupling mechanism. The structure is worth looking at closely. Adenine sits on one end, ribose in the middle, and the triphosphate tail on the other. The negative charges on the phosphate groups repel each other, creating electrostatic tension that contributes to the high negative Gibbs free energy change upon hydrolysis. That tension is relieved when the terminal bond breaks. The cell does not "burn" ATP like fuel. It transfers phosphate groups or exploits conformational changes in proteins that bind and hydrolyze ATP simultaneously. Most students miss how ATP regeneration works. The total amount of ATP in a typical human body at any moment is roughly 250 grams. You recycle your entire ATP supply somewhere between 1,000 and 1,400 times per day. That means around 50 to 70 kilograms of ATP are synthesized and consumed daily. The molecule itself is stable enough to store briefly but reactive enough to release energy on demand when the right enzyme positions it correctly.
I ran into a real problem once while putting together a problem set on oxidative phosphorylation. I needed students to calculate the P/O ratio for NADH under conditions where the proton leak was significant. The textbook values assumed perfect coupling, so the numbers never matched any realistic experimental data. I ended up pulling the actual numbers from the literature instead. With a proton leak of about 20 percent, the effective P/O ratio for NADH drops from the theoretical 2.5 to closer to 2.0. For FADH2 it drops from 1.5 to roughly 1.2. Including this in the problem set forced students to confront the difference between idealized chemistry and what actually happens in a living mitochondrion. The citric acid cycle produces one GTP per turn, which is functionally equivalent to ATP through nucleoside diphosphate kinase. That enzyme transfers the phosphate from GTP to ADP, generating GDP and ATP in a single step. Some curricula treat this as a minor detail. It is not. It matters when you are tracking the actual yield of phosphorylation events versus the number of direct ATP molecules synthesized. Another thing that trips people up is the difference between substrate-level phosphorylation and oxidative phosphorylation. Substrate-level phosphorylation happens directly during metabolic reactions, like when phosphoenolpyruvate donates a phosphate to ADP via pyruvate kinase in glycolysis. Oxidative phosphorylation depends on the electron transport chain and the proton gradient across the inner mitochondrial membrane. Both produce ATP, but the mechanisms and energy yields are completely different. Mixing them up on an exam is a fast way to lose points.
Get the Full Details
The chemiosmotic theory explains the oxidative phosphorylation mechanism. Electron transport through complexes I through IV pumps protons from the matrix into the intermembrane space. Complex V, or ATP synthase, allows protons to flow back into the matrix and uses that flow to rotate its internal components, driving the conversion of ADP and phosphate into ATP. The rotation speed matters. Each complete turn of the c-ring synthesizes three ATP molecules, and the number of c-subunits varies between species. In mammals it is eight, meaning eight protons are needed per ATP synthesized, plus additional protons for phosphate transport and ADP-ATP exchange through the adenine nucleotide translocase. Here is a counter-intuitive point that rarely gets emphasized: ATP is not the only nucleotide triphosphate cells use. GTP, CTP, UTP, and TTP all serve specialized roles. GTP powers protein synthesis at the ribosome. UTP activates glucose for glycogen synthesis. CTP is required for phospholipid production. The cell maintains these separately because the enzymes that use them are specific. You cannot swap GTP into an ATP-dependent reaction and expect the same outcome. The kinase that regenerates GTP from GDP is a different enzyme with different regulation. When ATP levels drop, AMP rises. AMP-activated protein kinase, or AMPK, senses this change and shifts the cell toward catabolic pathways while inhibiting anabolic ones. This is how cells sense energy stress. Cancer cells often have dysregulated AMPK signaling, which is one reason it gets studied so much in oncology research. Metformin, a common diabetes drug, works partly by activating AMPK through mild inhibition of complex I in the electron transport chain. The connection between ATP depletion and cellular signaling is more direct than most introductory courses convey.
There are scenarios where the ATP definition breaks down entirely. In some archaea and certain bacteria, alternative energy carriers exist alongside or instead of ATP. Some organisms use polyphosphate granules for energy storage. Others rely on thioesters or reduced ferredoxin for key biosynthetic steps. Calling ATP the universal energy currency is a shorthand that works for eukaryotes and most bacteria but does not cover every known biochemistry on Earth. That is worth noting when you encounter questions about extremophiles or alternative metabolic pathways. The practical takeaway is that ATP should be understood as a timing and transfer device, not a long-term energy store. Fat and glycogen are long-term stores. ATP is immediate. It sits in the cytoplasm and organelles waiting for an enzyme to position it for hydrolysis or transfer. The cell keeps the concentration of ATP high relative to ADP, typically around a 10-to-1 ratio, so that even small increases in demand can be met quickly without waiting for regeneration pathways to catch up. If you are studying this for an exam, focus on the coupling mechanism, not just the structure. Know how the phosphate transfer works, why the hydrolysis is favorable, and how the proton gradient ties back to the electron transport chain. The details about AMPK, the P/O ratios, and the c-ring stoichiometry will separate a solid grade from a mediocre one. The rest is vocabulary.