Working with Two Traits at Once
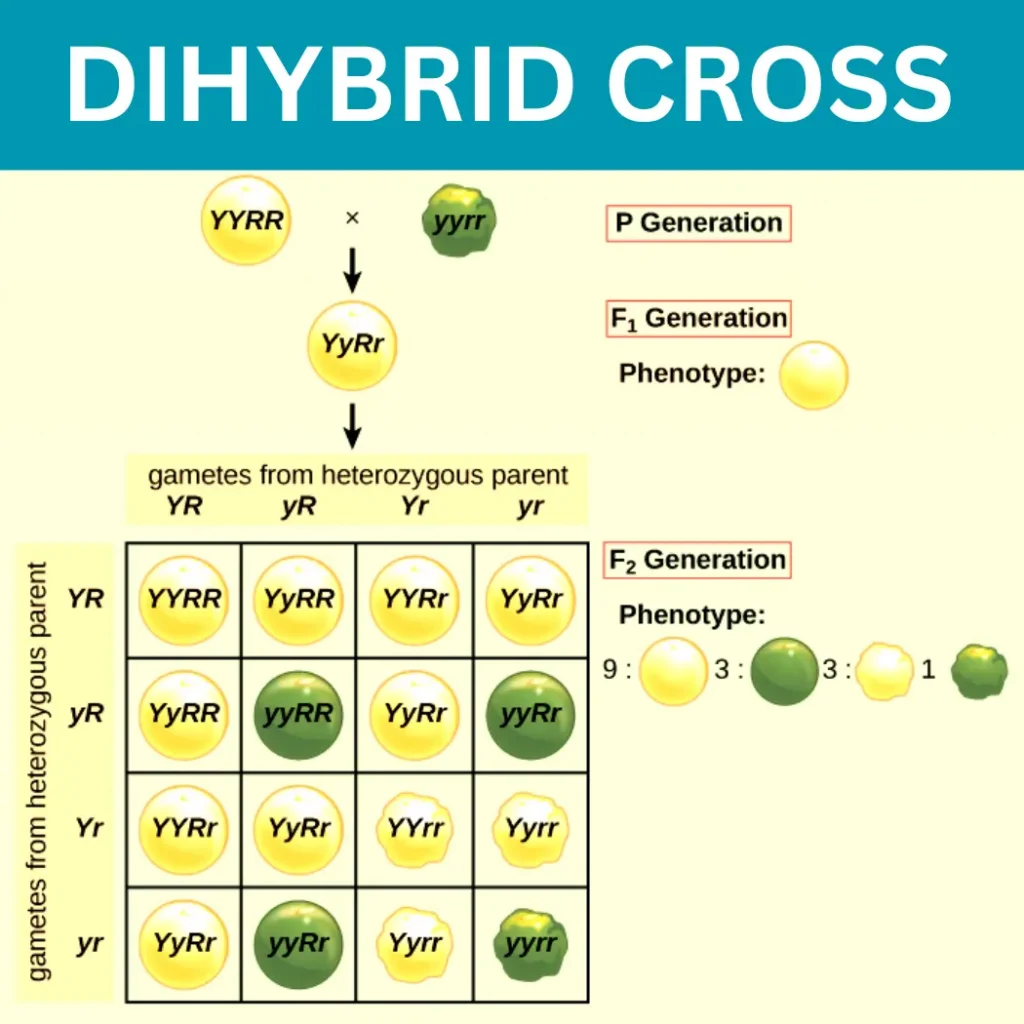
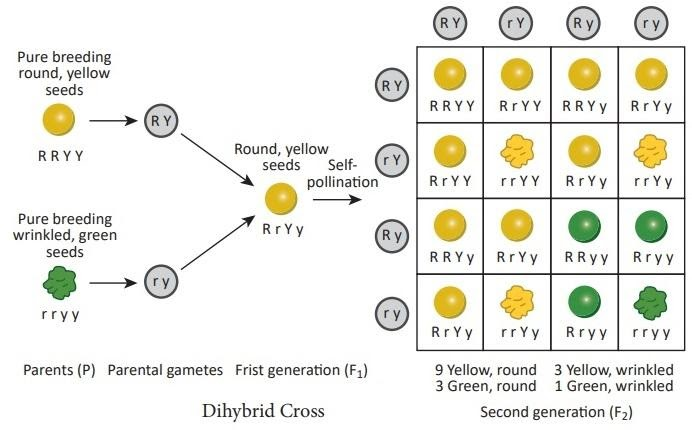
The easiest way to get confused about dihybrid crosses is to start with the definitions instead of the actual Punnett square grid. I used to do that in every genetics lab and waste about twenty minutes every time. The method itself is simple once you stop treating it like a different topic from monohybrid work. You just track two traits together and multiply the probabilities from each individual cross. A dihybrid cross tracks inheritance for two different genes simultaneously. Both parents are heterozygous for both traits, so the standard cross is AaBb × AaBb. The phenotypic ratio you see in the F2 generation is 9:3:3:1 when the genes assort independently. That is the baseline you build everything on. If the ratio looks different, something else is going on with linkage or epistasis. The genotype breakdown is messier. You get sixteen possible combinations in the full square. The phenotypes cluster into four groups: dominant for both traits, dominant for the first and recessive for the second, recessive for the first and dominant for the second, and recessive for both. Students often mix up which 3 belongs to which trait when they first draw it out.
Building the Square Step by Step
Start by determining what gametes each parent can produce. An AaBb parent makes four types of gametes: AB, Ab, aB, and ab. You get those by taking one allele from each gene. The FOIL method works if you want a mnemonic, but honestly it is just systematizing what you already know about meiosis. Each gamete gets one copy of gene A and one copy of gene B. Draw a 4×4 grid. Put one parent's gametes across the top and the other's down the side. Fill in each box by combining the alleles from the corresponding row and column. You end up with sixteen cells. Count the phenotypes in those cells and you should see nine showing both dominants, three showing dominant A with recessive b, three showing recessive a with dominant B, and one showing both recessives. The math shortcut is faster once you get comfortable. Instead of drawing the whole square, you can multiply the probabilities from each single-gene cross. Aa × Aa gives you 3/4 dominant and 1/4 recessive. Bb × Bb gives the same split. Multiply across: 3/4 × 3/4 = 9/16 for both dominant, 3/4 × 1/4 = 3/16 for the first dominant and second recessive, and so on. This cuts the process down from about five minutes of drawing to maybe thirty seconds of calculation.
The Edge Case I Ran Into
I was grading lab reports last semester and noticed one student consistently got 12:4:0:0 instead of 9:3:3:1. She thought she had done everything right. The actual problem was that she was looking at a test cross, not a dihybrid cross. A test cross uses AaBb × aabb, which gives a 1:1:1:1 ratio, not the classic F2 pattern. The confusion happens because some textbooks present both without clearly separating the scenarios. Another thing that trips people up is assuming independent assortment when the genes are actually linked. If two genes sit close together on the same chromosome, you will not get the expected ratios. The recombinant classes show up less frequently than the parental classes. I had a student who spent an entire lab period convinced she made arithmetic errors because her observed data was 7:1:1:7 instead of 9:3:3:1. The genes were linked about fifteen map units apart. It takes actual crossing data to confirm linkage, not just a single Punnett square prediction.
Get the Full Details

When This Approach Breaks Down
The 9:3:3:1 ratio only holds when two conditions are met: the genes must be on different chromosomes or far enough apart on the same chromosome to assort independently, and there can be no epistatic interactions between the loci. If gene A masks the expression of gene B, you get modified ratios like 9:3:4 or 12:3:1 instead. That is epistasis, and it is extremely common in actual biological systems even though textbook problems usually pretend it does not exist. Another limitation is sample size. The ratios are probabilistic, so small crosses rarely match the expected numbers exactly. A family with only four children might not show the classic distribution at all. You need larger sample sizes, usually several hundred offspring in experimental crosses, to see the ratio hold reliably. Some introductory courses skip over this point entirely, which leaves students thinking the 9:3:3:1 ratio is a hard rule rather than a statistical expectation.
Practical Notes on Dihybrid And Dihybrid Cross
Using the probability method instead of drawing full squares saves time and reduces transcription errors, but it does not help you visualize what is actually happening during fertilization. I recommend drawing at least one full 4×4 grid by hand before switching to multiplication. It takes about four minutes and makes the gamete combinations feel more concrete. After that, the shortcut is reliable. If you need a reference for practice problems, the Khan Academy genetics section has a worked example that follows the standard approach. For a deeper dive into deviations from expected ratios, Griffiths' Introduction to Genetic Analysis covers epistasis and linkage in detail. The dihybrid cross itself is usually in chapter three alongside the monohybrid material. The core idea you should walk away with is that a dihybrid cross is just two monohybrid crosses happening at the same time. The math stacks multiplicatively. The 9:3:3:1 pattern is a useful baseline for teaching, but real genetics rarely stays that clean. Expect deviations when you move past controlled textbook problems.