What You Actually Need to Know About Energy in Biological Systems
Most people walk into biology class thinking energy is just "what powers living things." That's not wrong, but it's useless when you're actually trying to work with it. The real definition you need to carry around is that energy in biology is the capacity to do work against thermodynamic constraints within an aqueous, room-temperature environment. Everything else is just the messy details of how cells handle that problem. When I first started working with metabolic modeling, I ran into a wall where the textbooks and the lab data just didn't line up. The problem was stoichiometric models treating ATP hydrolysis as a simple exergonic reaction with a fixed delta G of negative 30.5 kilojoules per mole. That value assumes standard conditions — one molar concentrations, pH seven, twenty-five degrees Celsius. Living cells don't exist under standard conditions. They exist at millimolar or micromolar concentrations, pH varies between compartments, and temperature fluctuates. I spent about three weeks trying to get my flux balance analysis to match actual respiration rates before I realized the issue was thermodynamic context, not model structure. The workaround was calculating actual Gibbs free energy using the equation delta G equals delta G naught plus R T ln of Q, where Q is the reaction quotient based on actual intracellular concentrations. I pulled concentration data from public metabolite databases and built a correction layer into the model. The difference between standard-state and actual-state energy values for key reactions like phosphoglycerate kinase and pyruvate kinase was substantial enough to flip predicted flux directions entirely. That changed how I approach every energy calculation since.Energy Definition In Biology: The Practical Breakdown
Let's start with the mechanism before we get to definitions, because definitions made sense only after I understood what's actually happening at the molecular level. Biological energy transfer is almost entirely mediated through phosphorylation. ATP donates a phosphate group to another molecule, and that transfer is coupled to work — whether that's mechanical work like myosin walking along actin, transport work like the sodium-potassium pump moving ions against gradients, or chemical work like driving endergonic reactions forward. The phosphate bond isn't special because it stores a huge amount of energy. It's special because the hydrolysis products are dramatically more stable than the reactants, and that stability difference is what gets channeled into useful work. Here's the part most introductions skip. Energy in biological systems is not a substance. You can't isolate it, bottle it, or measure it directly the way you measure mass or volume. What you can measure are energy transformations — heat released, bonds broken and formed, ion gradients established, concentrations changed. Every definition you encounter is really describing a bookkeeping method for tracking those transformations through biological processes. The thermodynamic framework is non-negotiable here. First law, energy is conserved. Second law, entropy increases in any real process. Biology doesn't violate either law. What it does is create local order by exporting disorder to the surroundings, which is why cells need a constant energy input. A resting human being dissipates roughly one hundred watts of power as heat while maintaining internal organization that would be thermodynamically unlikely without that input. That's not poetry, that's just basic thermodynamics applied to a warm-blooded animal.
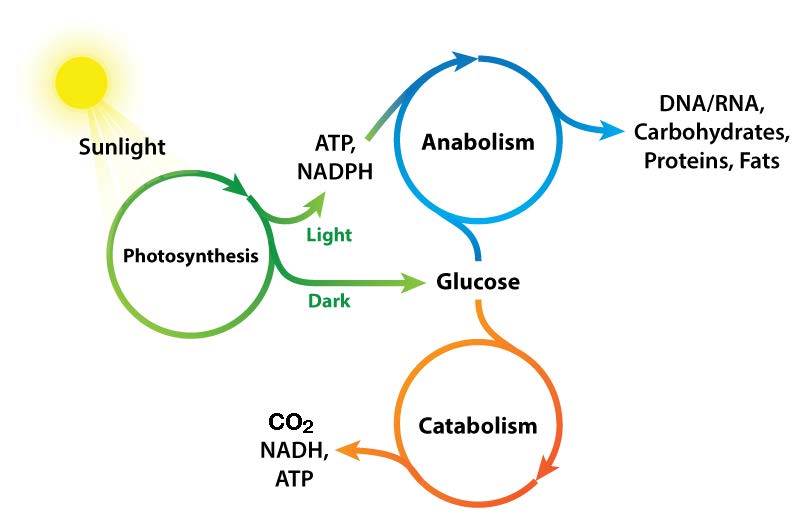
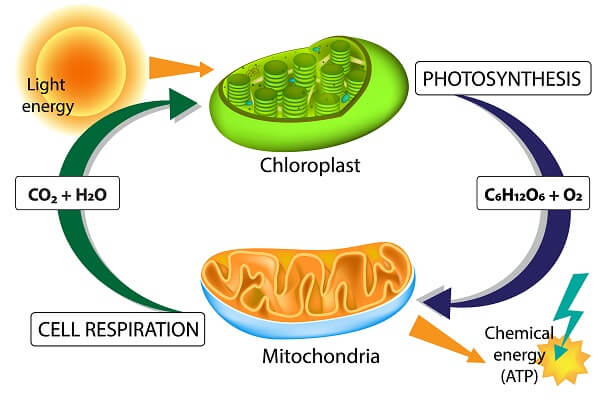
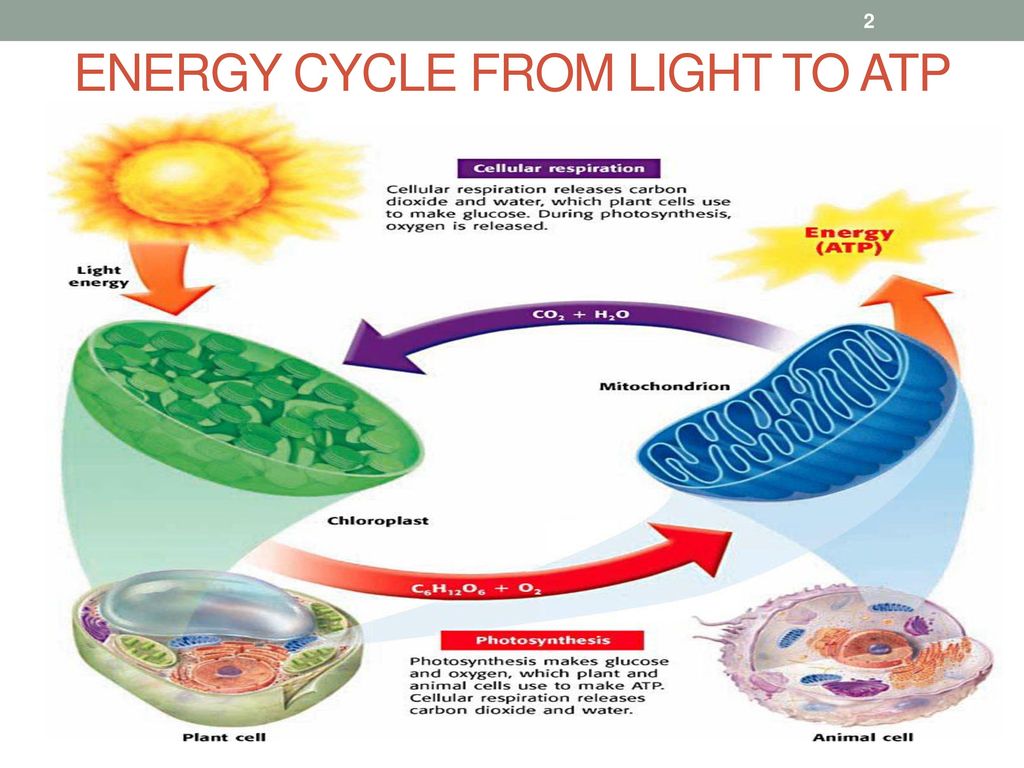
When you're working with actual biological energy data, you'll encounter three main energy currencies that matter. ATP is the immediate donor, NADH and NADPH carry reducing equivalents that represent stored electron energy, and proton motive force is the electrochemical gradient that drives ATP synthesis and other work. These three are interconnected through oxidative phosphorylation and photosynthesis, and confusing them or treating them as independent is a common beginner mistake. Proton motive force especially gets underestimated. It's not just an intermediate step to making ATP. It directly powers flagellar rotation, nutrient uptake through symporters, and heat generation in brown adipose tissue. If your analysis only accounts for ATP, you're missing significant energy flows. The enthalpy and entropy contributions to biological reactions also deserve attention that they don't usually get. Enthalpy tells you about bond energies and heat exchange. Entropy tells you about disorder and the dispersal of energy. In aqueous biological systems, hydrophobic effects drive massive entropy changes that power protein folding, membrane formation, and substrate binding. When I model ligand-receptor interactions, I've seen binding events where the enthalpy change is unfavorable but the entropy change is so large and positive that the overall free energy is strongly favorable. The binding is driven by water displacement, not by attractive forces between the molecules. Beginners often look at enthalpy alone and conclude a reaction shouldn't happen, when entropy is doing all the actual work. There's a practical measurement issue that comes up whenever you try to apply these concepts to experimental data. Calorimetry gives you total heat output, which relates to enthalpy change, but it doesn't tell you how that energy is partitioned among different processes. Respirometry gives you oxygen consumption or carbon dioxide production, which relates to electron flow and ATP production rates, but it requires assumptions about P-O ratios and coupling efficiency that aren't always valid. I've seen papers report ATP production rates that are off by a factor of two because they assumed perfect coupling between electron transport and ATP synthesis when the system was actually partially uncoupled. Uncoupling proteins are widespread — they're not pathological exceptions. They're present in mitochondria, in plastids, and in bacterial membranes under normal physiological conditions.
Another area where definitions break down in practice is the concept of energy charge. Atkinson's energy charge formula — plus ATP and half of ADP divided by the total adenine nucleotide pool — gives you a single number between zero and one that represents the energetic status of a cell. The useful range for most living cells is around zero point eight. Below that, growth stops. Above that, the cell is in an energetically privileged state that usually indicates pathology or artifact. I've encountered cases where researchers measured adenine nucleotides but didn't calculate energy charge, and they missed a key regulatory signal because they were looking at absolute concentrations instead of the ratio that actually matters for enzyme kinetics. Many glycolytic and biosynthetic enzymes are allosterically regulated by energy charge, not by the concentration of any single nucleotide. When you're defining energy for a specific biological context, the definition needs to match the scale you're working at. Cellular energy metabolism has different constraints than tissue-level energy allocation, which has different constraints than ecosystem-level energy flow. Trophic efficiency in ecosystems follows the roughly ten percent rule, but that's a statistical approximation that varies widely depending on whether you're looking at marine plankton or terrestrial herbivores. The inefficiency comes from respiration, waste, and unconsumed biomass, not from any single mechanism. Understanding where the energy actually goes at each level prevents you from applying ecosystem-level rules to cellular problems or vice versa. One more thing that causes problems in real work. People conflate energy with power. Energy is a quantity. Power is the rate of energy transfer. A cell might have enough energy stored in its ATP pool to sustain activity for a few seconds, but the power — the rate at which it can regenerate that ATP — determines what the cell can actually do in real time. Sprinting versus endurance running in muscle tissue is fundamentally a difference in power output capacity, not total energy content. The same applies at the cellular level. Cancer cells often have high glycolytic flux because they need power, not because they're inefficient. They're optimizing for rate over yield, which is a completely rational choice when growth speed matters more than energy conservation.
Get the Full Details