Understanding How Natural Selection Actually Works In Practice
Natural selection is one of those concepts everyone learns in high school biology, but very few people actually understand what it means when you're standing in the field trying to measure it. The textbook version is straightforward: individuals with certain heritable traits survive and reproduce better than others, so those traits become more common over generations. The reality of working with it is messier, slower, and often frustratingly indirect. The most reliable example you can point to without getting into debate territory is the case of industrial melanism in the peppered moth. Before the Industrial Revolution in England, the light-colored form of Biston betularia dominated because it blended with lichen-covered tree bark. Dark-colored moths were rare because birds could spot them easily. As coal pollution killed the lichen and blackened the trees, the dark form became camouflaged and the light form stood out. Within about fifty years, the population shifted dramatically. When clean air legislation was passed later, the trend reversed. This is not speculation. It was documented with actual trapping data by researchers like Kettlewell and subsequently by many others across multiple decades. Here is what makes that example work well for demonstration purposes. The trait is clearly defined, visible to the naked eye, and directly tied to predation risk. The environmental change is independent of the moth population itself. The shift happened fast enough to be observed within a human lifetime rather than over millions of years. Most field examples of natural selection lack that kind of clarity.
What You Actually Need To Show Or Demonstrate This
If you are putting together educational material or trying to show someone how natural selection operates in real time, you need three things: a trait that varies between individuals, a mechanism that makes that variation affect survival or reproduction, and a way to track the change over time. Without all three, you are just describing evolution, not natural selection specifically. Evolution also covers genetic drift and gene flow, which operate through different mechanisms entirely. I have tried building classroom exercises around artificial selection with plants because it is faster and more visible. Sunflower seed size or pepper fruit heat level works well. But the moment someone asks whether that proves natural selection happens in the wild, the answer is no, it proves selection exists as a mechanism. The transfer requires you to then connect it back to a wild system, which is where most people get stuck.
The Anticipate-Measure-Confirm Workflow
When I work with this material, I structure it around a loop rather than a straight line. You start by identifying a population with measurable trait variation and a plausible environmental pressure. Then you predict which trait values should be favored under that pressure. After that, you collect data on survival or reproductive output across trait categories. Finally, you compare the observed shift to your prediction. If it does not match, you revise the mechanism rather than discard the whole framework. This approach usually takes about three to four weeks for a classroom setting using simulated organisms or quick-growing plants. Field studies take longer because natural systems do not follow a schedule. I have seen projects stall for a full semester because the environmental variable they needed to measure was seasonal and their timeline missed the window entirely. That is a practical bottleneck you need to plan around, not something theory tells you about.
Get the Full Details
Where Beginners Mess This Up
The most common error is treating natural selection as intentional. It is not. Organisms do not decide to adapt. Individuals do not change their genetics in response to pressure. The population changes because certain genotypes leave more offspring than others. Language matters here. Saying "the moths adapted to the pollution" is shorthand that reinforces the wrong mental model. A more accurate phrasing is that the polluting environment changed the relative fitness of existing color morphs, and allele frequencies shifted as a result. Another frequent problem is conflating correlation with selection. Just because a trait is more common in a certain environment does not mean natural selection caused it. The trait could be linked to another gene under selection, it could be a result of non-random mating, or the environment could be correlated with a third variable you have not measured. This is why controlled field studies or mark-recapture experiments exist. They are not glamorous, but they are the only way to separate selection from the noise.
One Edge Case That Always Comes Up
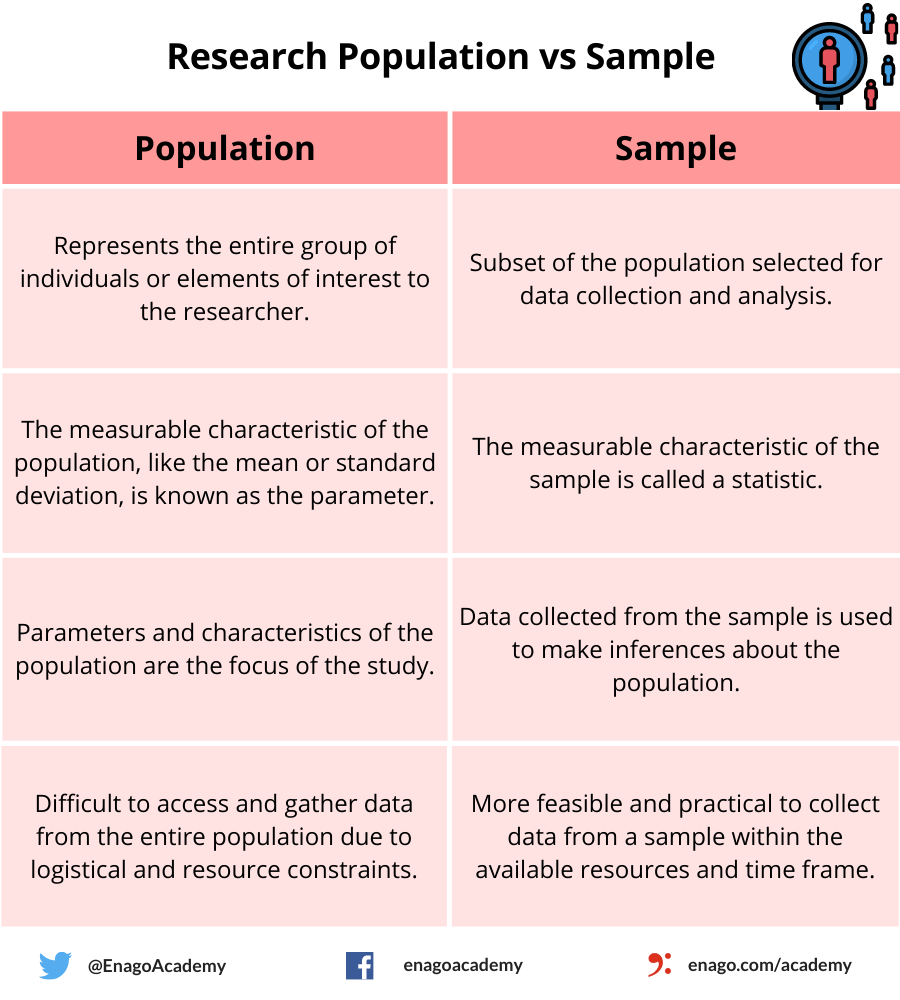
I ran into this while trying to document selection in a small population of urban birds. The trait I was tracking showed a clear frequency shift over two years, which initially looked like a strong selection signal. The problem turned out to be a severe bottleneck event that reduced population size by roughly seventy percent due to a construction project nearby. What I thought was directional selection was actually genetic drift acting on a small population. The workaround was straightforward: I had to collect neutral genetic markers to estimate effective population size and then run a comparison model that separated drift from selection coefficients. It added about a week of lab work and cost roughly four hundred dollars in genotyping, but it was the only way to avoid publishing a false result. This is why sample size and demographic history matter more than people admit when they first get excited about a trait shift. First, natural selection is not the only evolutionary force, and it is not always the strongest one. In small populations, drift can overwhelm selection entirely, especially for traits with small selective effects. Many published studies have overestimated the strength of selection because they did not account for this interaction. The standard formula for the threshold where drift dominates is when the effective population size multiplied by the selection coefficient is less than one. That number tells you immediately whether your observed change could plausibly be drift instead. Second, what looks like optimal adaptation is often constrained by trade-offs, pleiotropy, or historical contingency. A trait does not become perfect. It becomes good enough given the existing genetic toolkit and the current environment. There are well-documented cases where a mutation would improve fitness in isolation but cannot fix because it is linked to a deleterious allele on the same chromosome, or because the same gene controls multiple functions and changing it breaks something else. This is why studying natural selection without population genetics context leads to naive conclusions about design.
When Natural Selection Is Not The Right Explanation
If you are looking at a trait distribution and considering selection as the cause, check these conditions first. Is the trait heritable? Can you demonstrate that, or are you assuming it? Is there a mechanism linking the trait to fitness, or are you just observing a pattern and calling it selection? Is the population large enough that drift is unlikely to produce the observed shift? If you cannot answer the first question empirically, you do not have evidence of natural selection, regardless of how clean the pattern looks. For cases where heritability is unclear or the population is small, I recommend starting with common garden experiments or quantitative genetics approaches rather than jumping to selection coefficients. Field observations are useful for generating hypotheses, but they are weak evidence on their own. The distinction is not academic. It determines whether your conclusion holds up under peer review or gets torn apart in the first round of critique. The resources I consistently point to for working through this properly are the papers by Endler on the methods of studying natural selection in the wild and the quantitative genetics framework from Lynch and Walsh. They are dense, but they cover the statistical reality of measuring selection gradients, which most introductory material skips entirely. If you need a downloadable reference that summarizes the key equations and study designs in one place, the online appendices from those texts are freely available and save you from reconstructing the methods from scattered journal articles.


