Understanding Behavioral Adaptations Through Real Observation
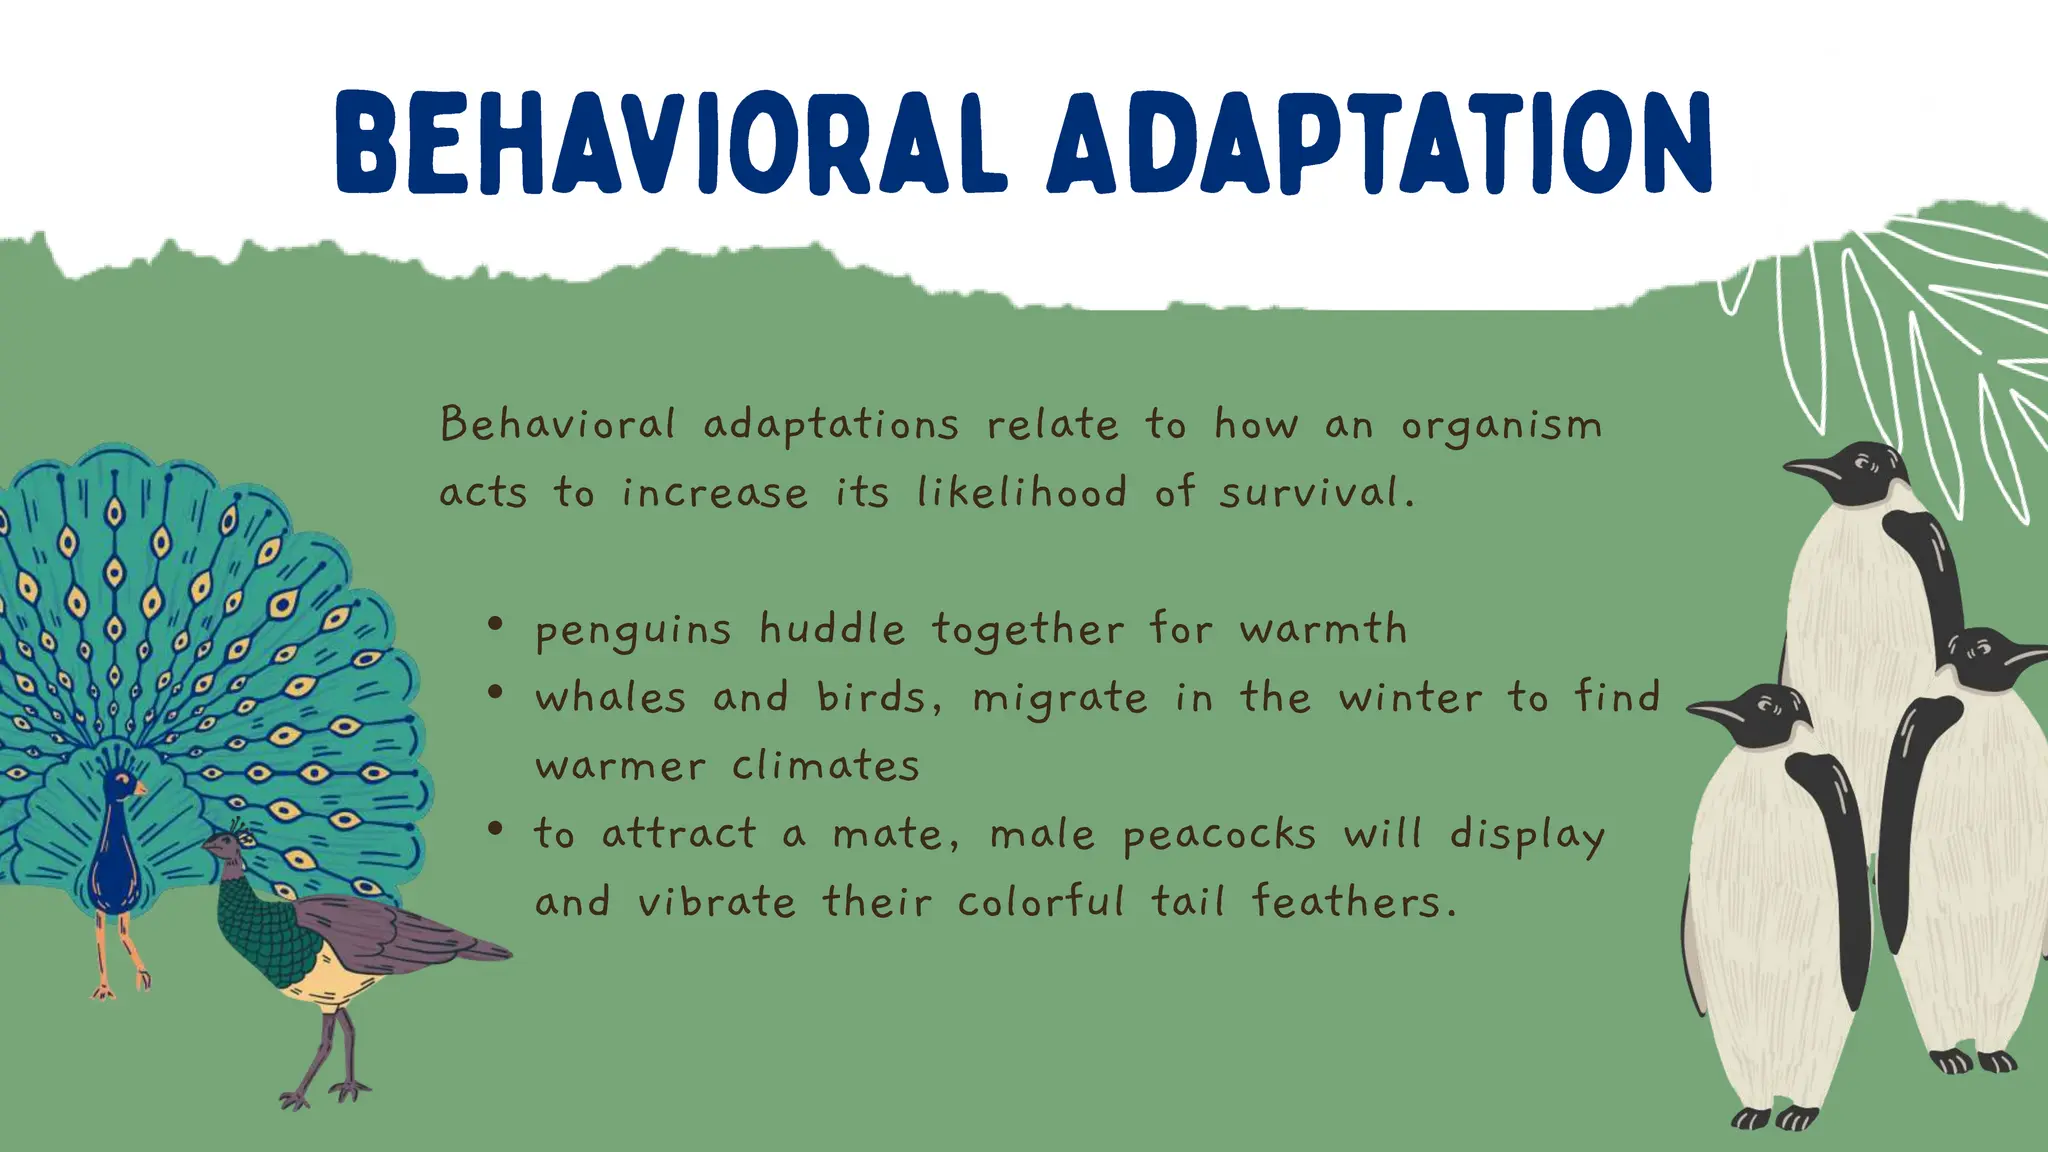
Behavioral adaptations are the learned or instinctive actions organisms take to survive and reproduce in their environments. They're distinct from structural or physiological adaptations because they involve what an animal does rather than what it looks like or how its body functions internally. When you're studying field biology or ecology, these become the most interesting category because they're observable in real time without needing to dissect anything. I spent three summers tracking nesting patterns in shorebird colonies along the Pacific coast, and what stood out immediately was how context-dependent behavioral adaptations are. A behavior that looks like a clear survival strategy in one situation can be completely maladaptive in another. For instance, many shorebird species perform what's called a "broken wing act" to lure predators away from their nests. You'll see an adult bird limping dramatically across the beach, apparently injured and easy prey. The predator takes the bait, and once it's far enough from the nest, the bird simply flies off. This behavior is genetically programmed in most populations, but here's the thing most textbooks don't mention: it only works reliably when the predator is a mammal or bird that relies on visual cues. I watched a single garter snake ignore the display entirely and just follow the sound of the bird's distress calls instead. The adaptation had failed, not because the behavior was wrong, but because the predator's sensory ecology didn't match the assumed threat model. This is the kind of edge case that comes up constantly when you're trying to categorize Examples Of Behavioral Adaptations for a course or research paper. The standard textbook examples — migration, hibernation, mating dances, parental care — are all valid, but they're almost too clean. Real organisms are messier. A prairie dog's alarm call system, for example, isn't just a simple signal for "predator." Different calls correspond to different predator types, sizes, and approaches. Researchers like Con Slobodchikoff demonstrated that the calls even encode information about the color and size of human intruders. That level of specificity wasn't predicted by any earlier model.
The key insight most beginners miss is that behavioral adaptations exist on a continuum between innate and learned. Some behaviors are fully hardwired, like the stickleback fish's mating dance triggered by the red belly of a rival male. Others are partially learned through trial and error, like the way young chimpanzees acquire termite-fishing techniques from their mothers. And then there are behaviors that appear to be culturally transmitted across groups with no genetic basis, like the potato-cleaning tradition of Japanese macaques that started with a single individual named Imo in 1953 and spread through the troop over roughly a decade. When you're evaluating whether a behavior qualifies as an adaptation at all, you need to ask whether it increases fitness relative to alternative behaviors in the same population. If the behavior is just a byproduct of something else — say, a bird's song that happens to attract mates because it correlates with brain size rather than being selected for directly — then you're looking at a spandrel, not an adaptation.
How to Identify Behavioral Adaptations Yourself
The practical method I use is straightforward but requires patience. First, document the behavior in detail: what triggers it, how often it occurs, who performs it, and what the immediate and delayed consequences are. Second, compare individuals that perform the behavior against those that don't. Are the performers producing more offspring? Surviving longer? Accessing better resources? Third, and this is where people usually cut corners, rule out alternative explanations. The behavior might correlate with survival without actually causing it. A classic example is the supposed courtship feeding behavior in spiders where the male presents the female with a wrapped prey item. The adaptationist explanation is that it reduces the risk of cannibalism during mating. But when researchers controlled for the female's hunger level, the protective effect largely disappeared. The behavior was real, but the adaptive function was overstated. I once spent two weeks trying to code the behavioral sequences of banded mongooses during cooperative breeding, and the data nearly broke my initial framework. Males and females both contribute to pup care, but the contribution patterns shifted dramatically depending on whether the litter was same-sex or mixed-sex. In same-sex litters, females did significantly more warming and provisionment. In mixed-sex litters, males compensated almost exactly. No single textbook example of behavioral adaptation captures this kind of flexible, condition-dependent response. The workaround was to stop treating the behavior as a fixed trait and instead model it as a decision rule: given the sex ratio of the litter and the number of available helpers, each individual adjusts its investment to maximize inclusive fitness. It took about six months of re-analysis before the pattern became clear, but once it did, it fit the predictions of Hamilton's rule almost perfectly.
Get the Full Details

Limits and When the Framework Breaks Down
Behavioral adaptation analysis has real limitations that worth being honest about. The biggest issue is the difficulty of measuring fitness directly. You can observe behavior for years without ever knowing whether it actually affected reproductive success. A deer's freezing response to a potential threat is obviously adaptive in theory, but proving it increased lifetime reproductive output requires mark-recapture data across multiple generations, which most researchers don't have. Another problem is the assumption of optimality. Behavioral ecologists often model organisms as if they're making rational cost-benefit calculations, but animals don't have access to the information their environment provides. A song sparrow defending territory doesn't know the precise energetic costs of singing versus fleeing. It follows rules of thumb shaped by selection, and sometimes those rules produce suboptimal outcomes in novel situations. Perhaps the most serious limitation is that behavioral plasticity can actually mask the absence of adaptation. If a species can adjust its behavior flexibly to almost any change in environment, then there's less selective pressure for fixed behavioral adaptations. This is called the Bambi Effect, and it means that behavioral flexibility might make it harder to detect true adaptations because the organism appears to be coping well across a wide range of conditions when in reality it's just switching responses. If you're studying a species with high behavioral plasticity, I'd recommend combining your behavioral observations with physiological or genetic data to triangulate whether a behavior is truly adapted or just flexible. The takeaway isn't that behavioral adaptations aren't real or important. They absolutely are, and they're often the most visible and fascinating aspect of how organisms interact with their world. The point is that identifying them requires careful, multidimensional evidence. Good examples exist — the waggle dance of honeybees conveying spatial information about food sources, the salmon's homing instinct using olfactory imprinting, the burrowing owl's strategy of using snake deterrents by mimicking rattlesnake sounds — but each one holds up only under scrutiny. When you encounter a claimed behavioral adaptation, ask what the alternative hypotheses are, what the fitness data shows, and whether the behavior would still make sense if the ecological context shifted slightly. That's how you separate genuine adaptations from convenient stories.