Understanding Trophic Energy Flow in Real Ecosystems
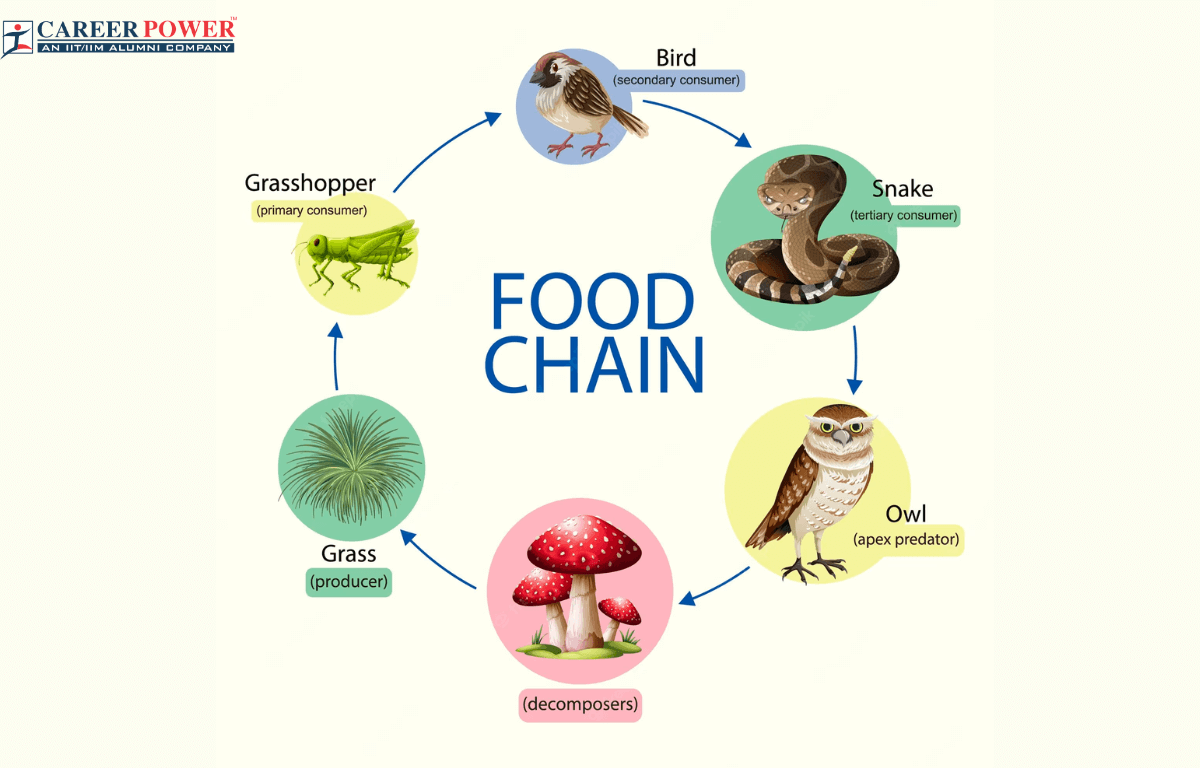
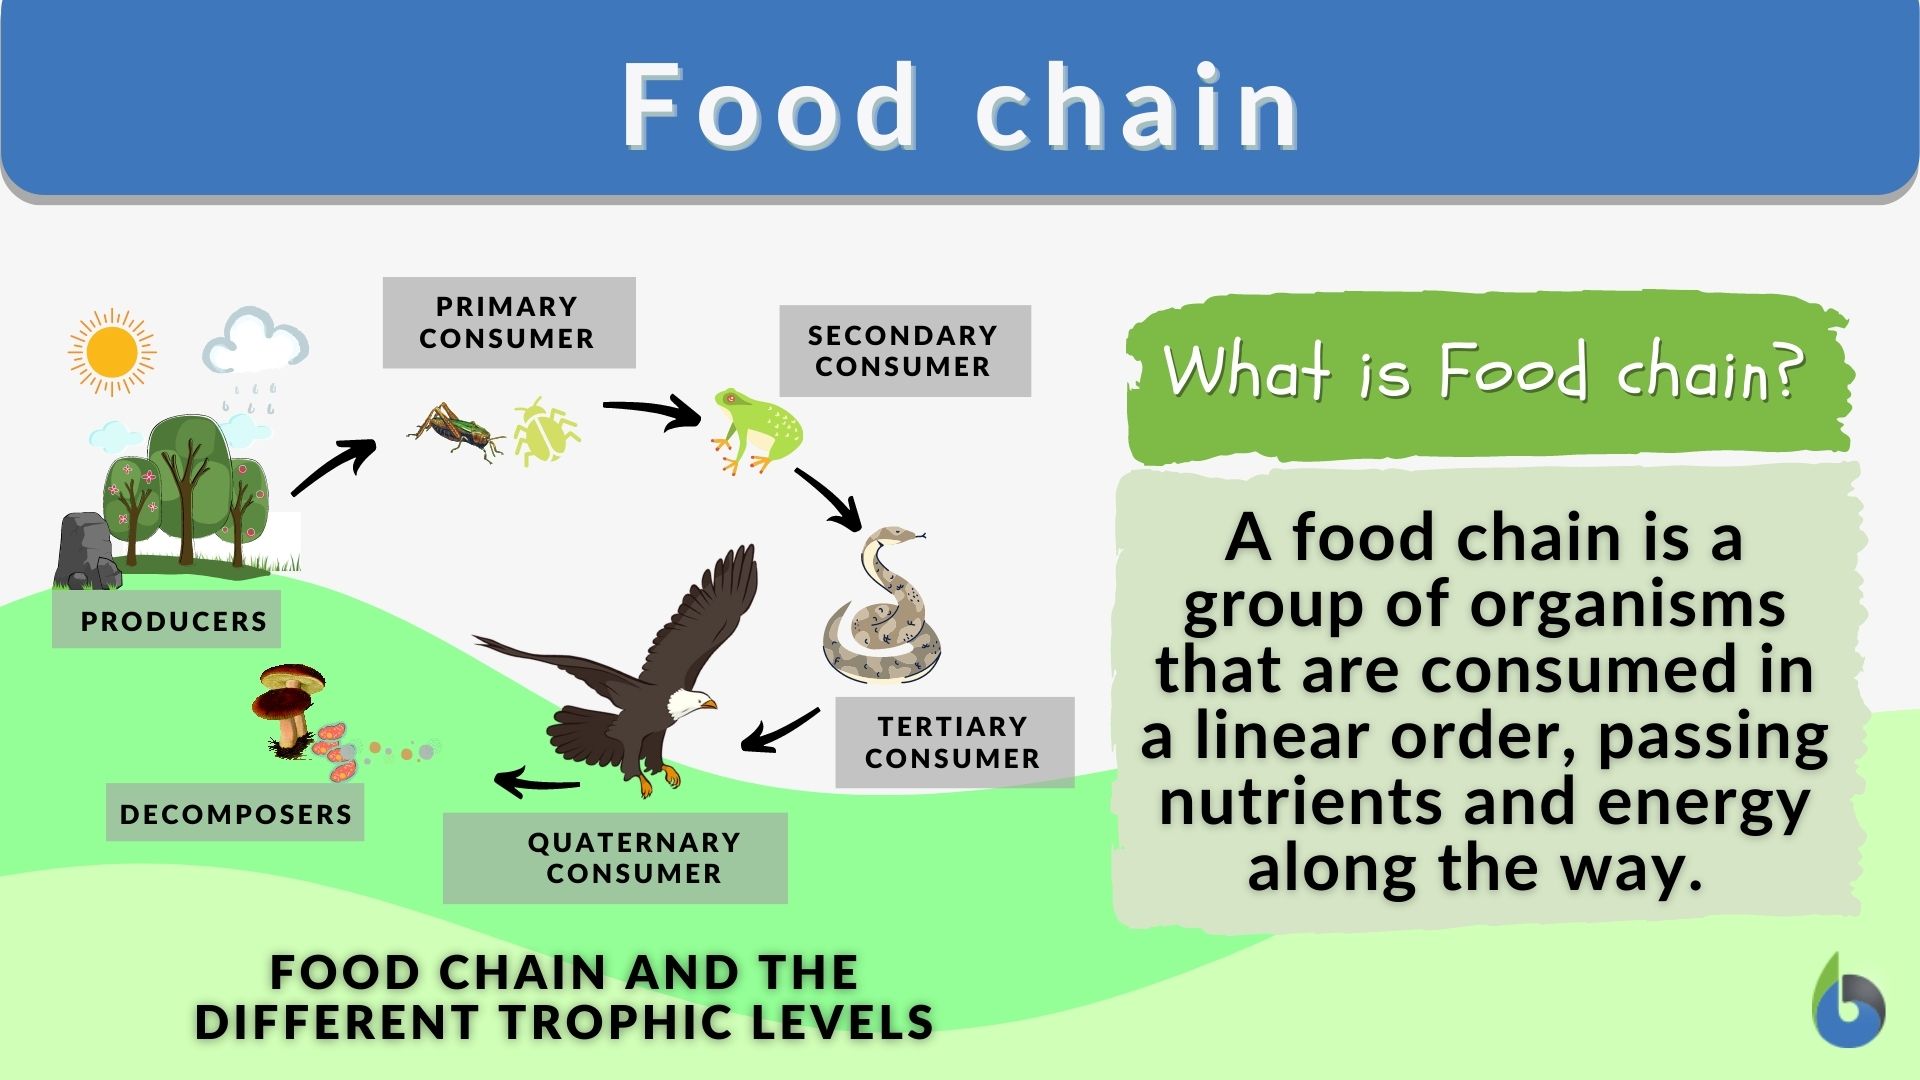
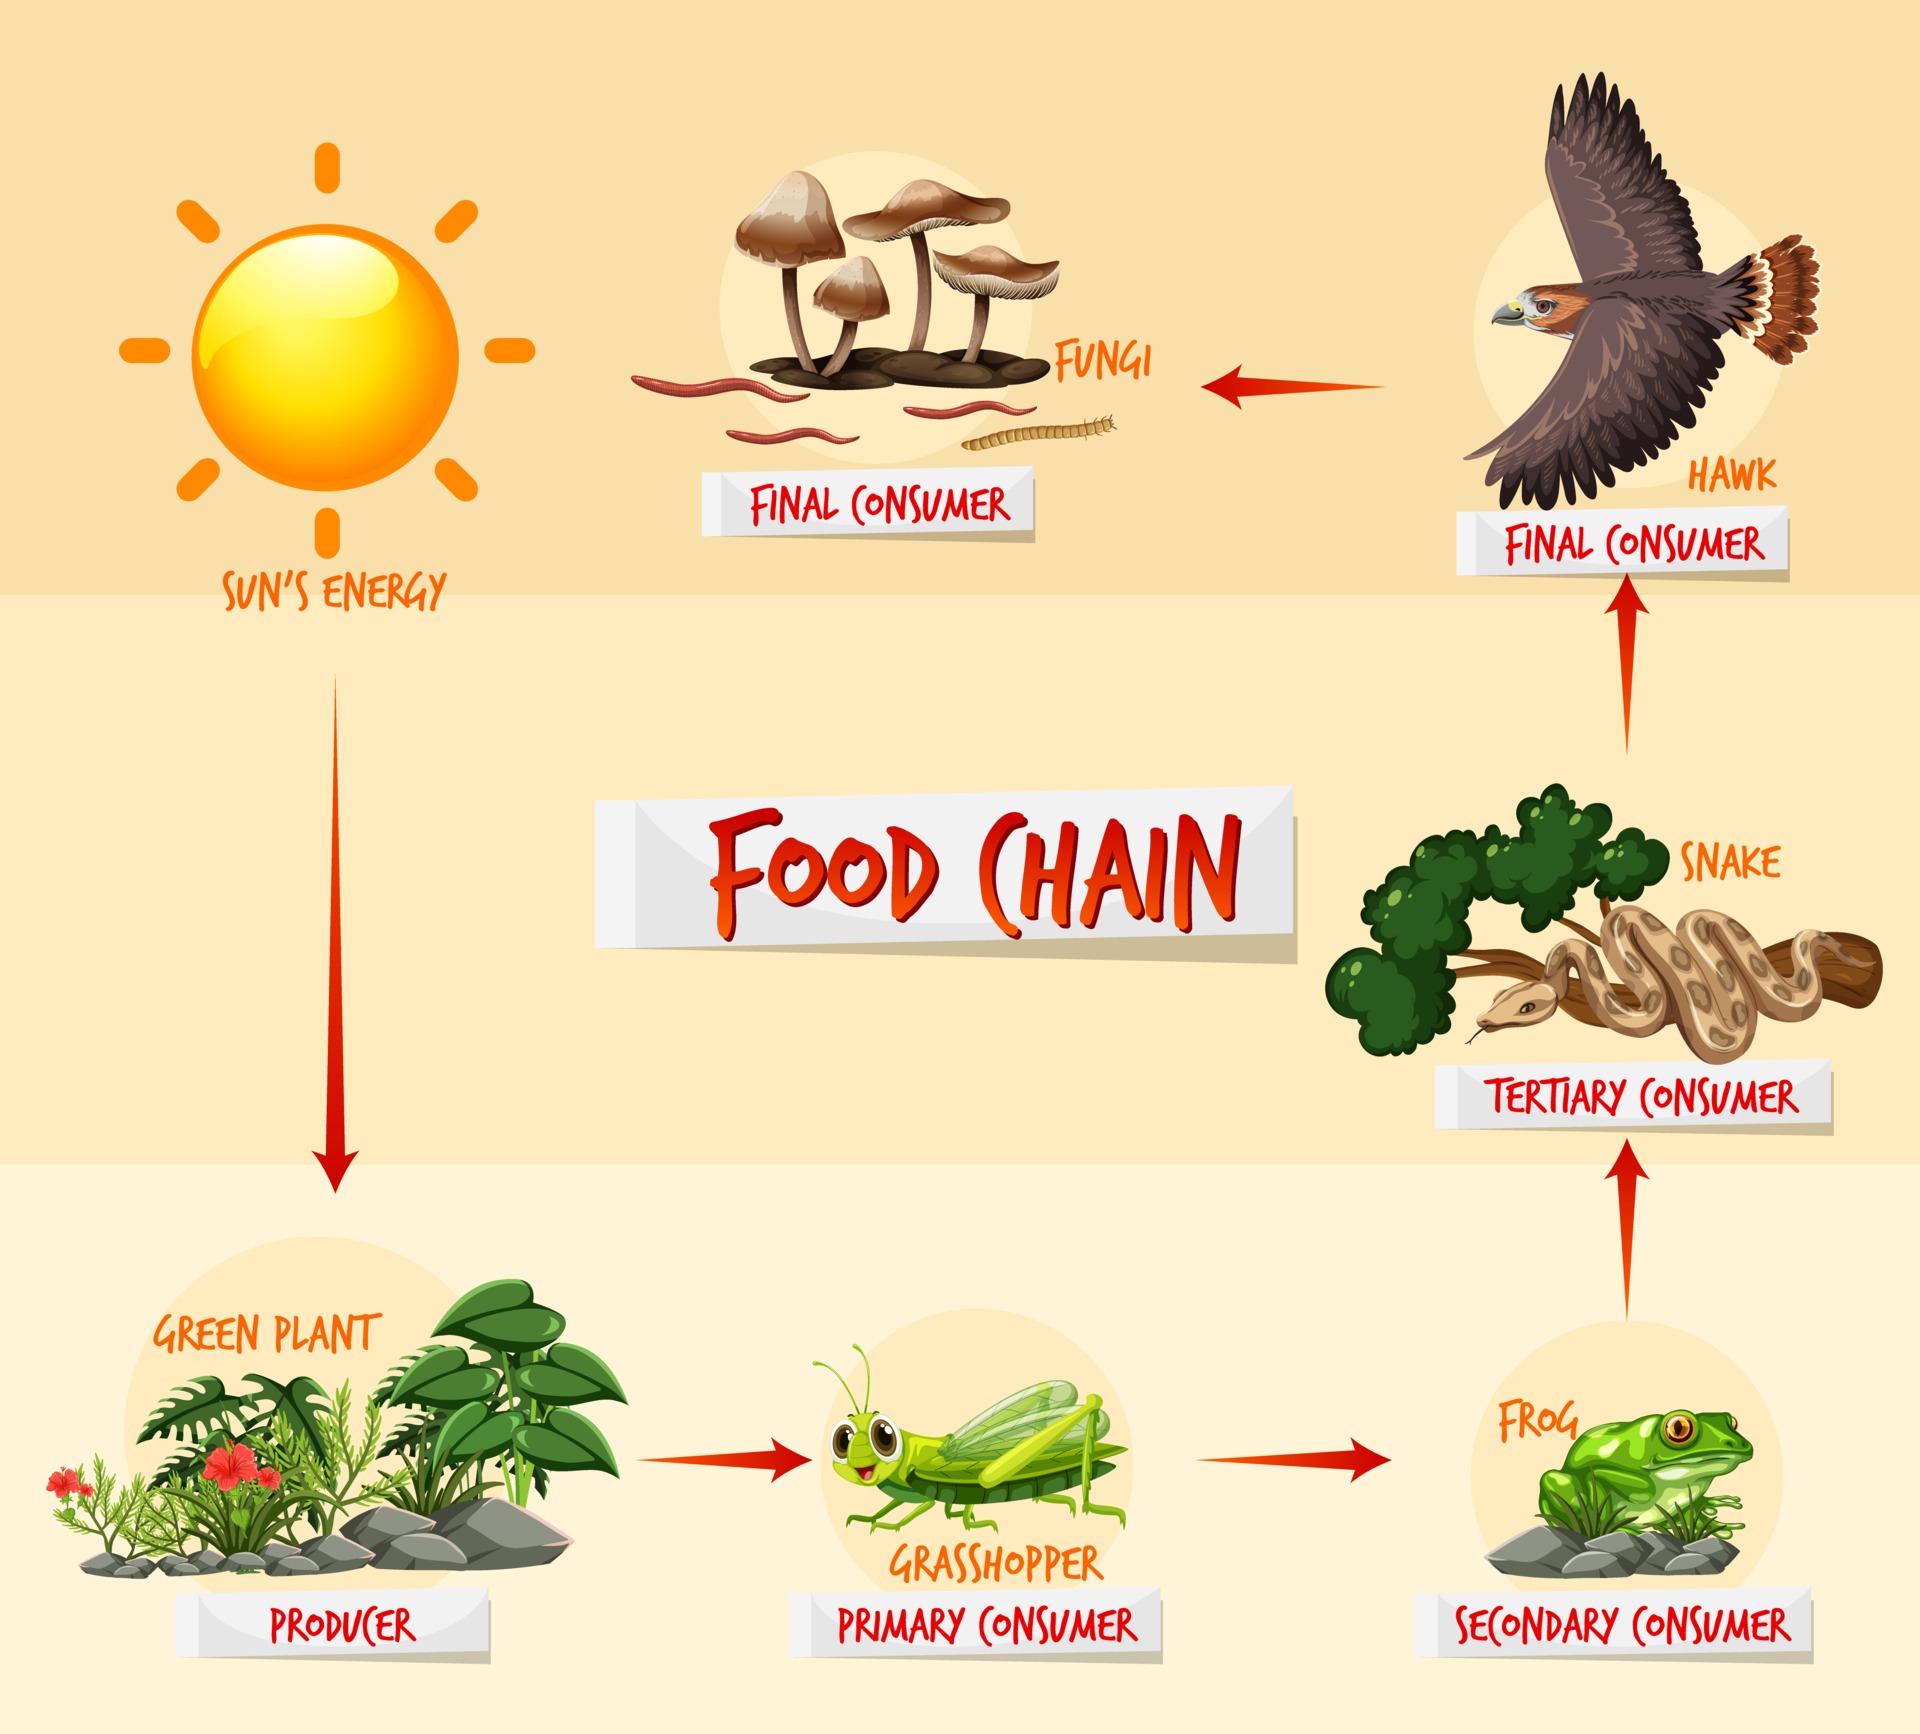
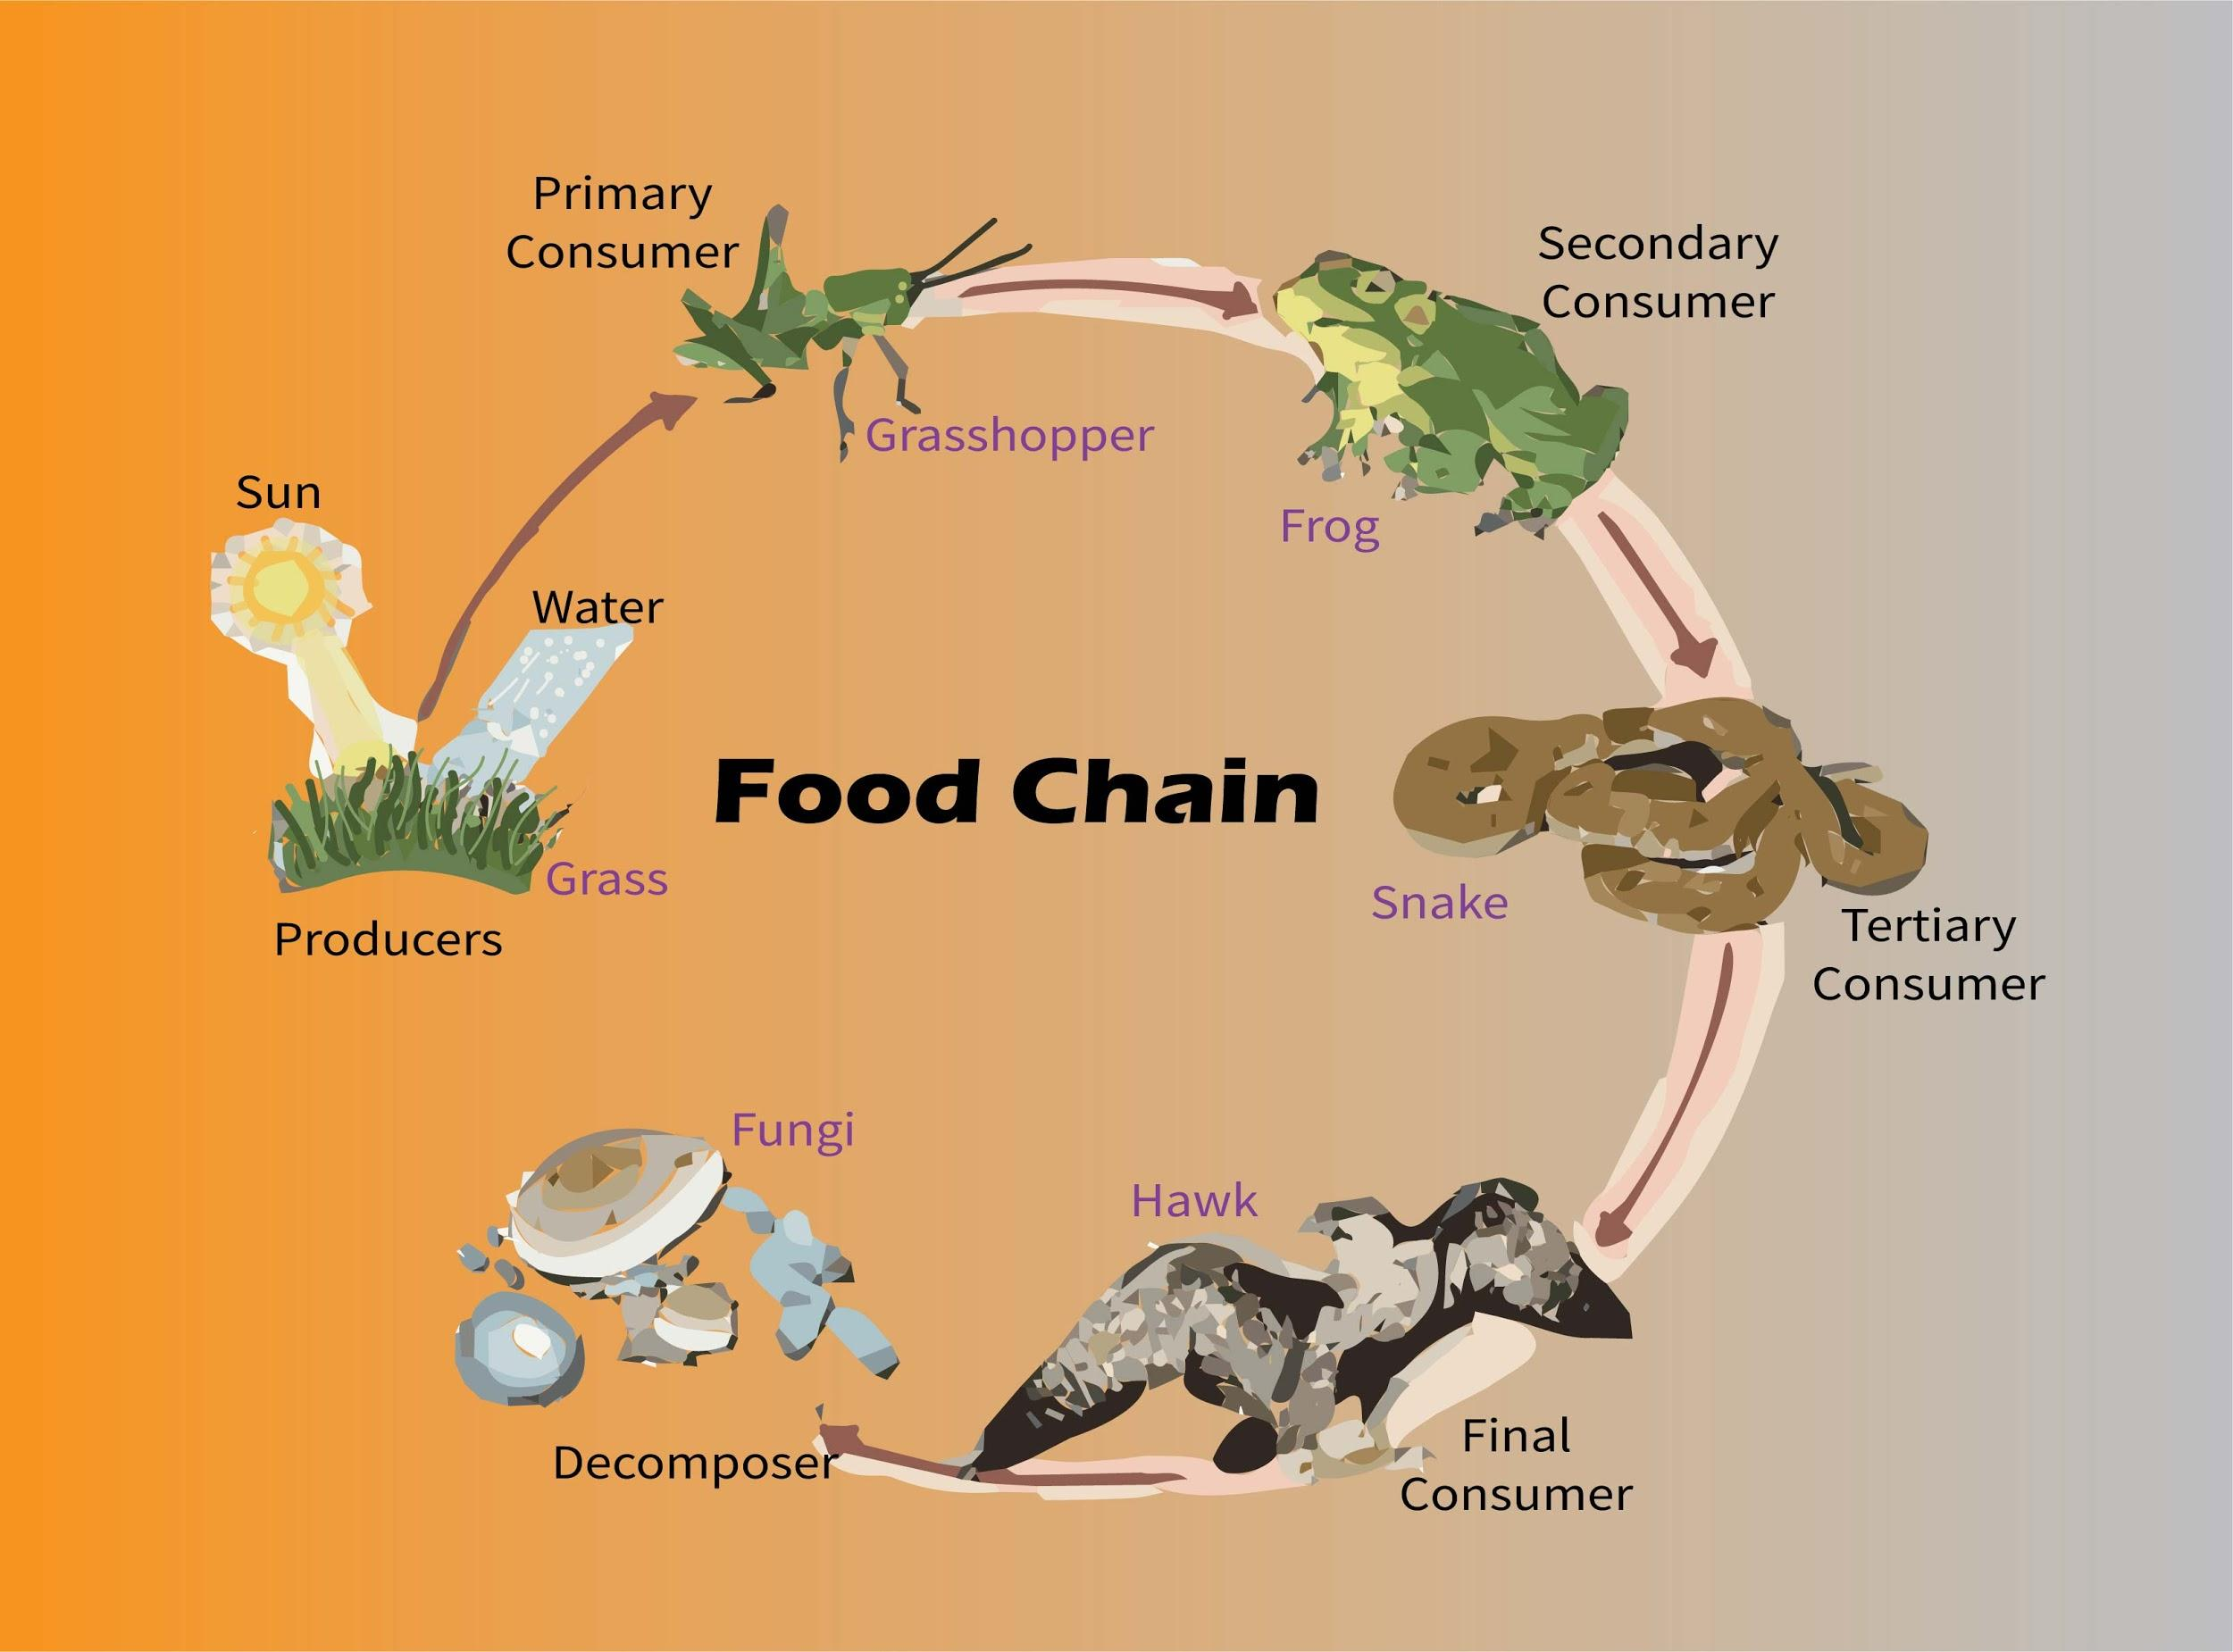
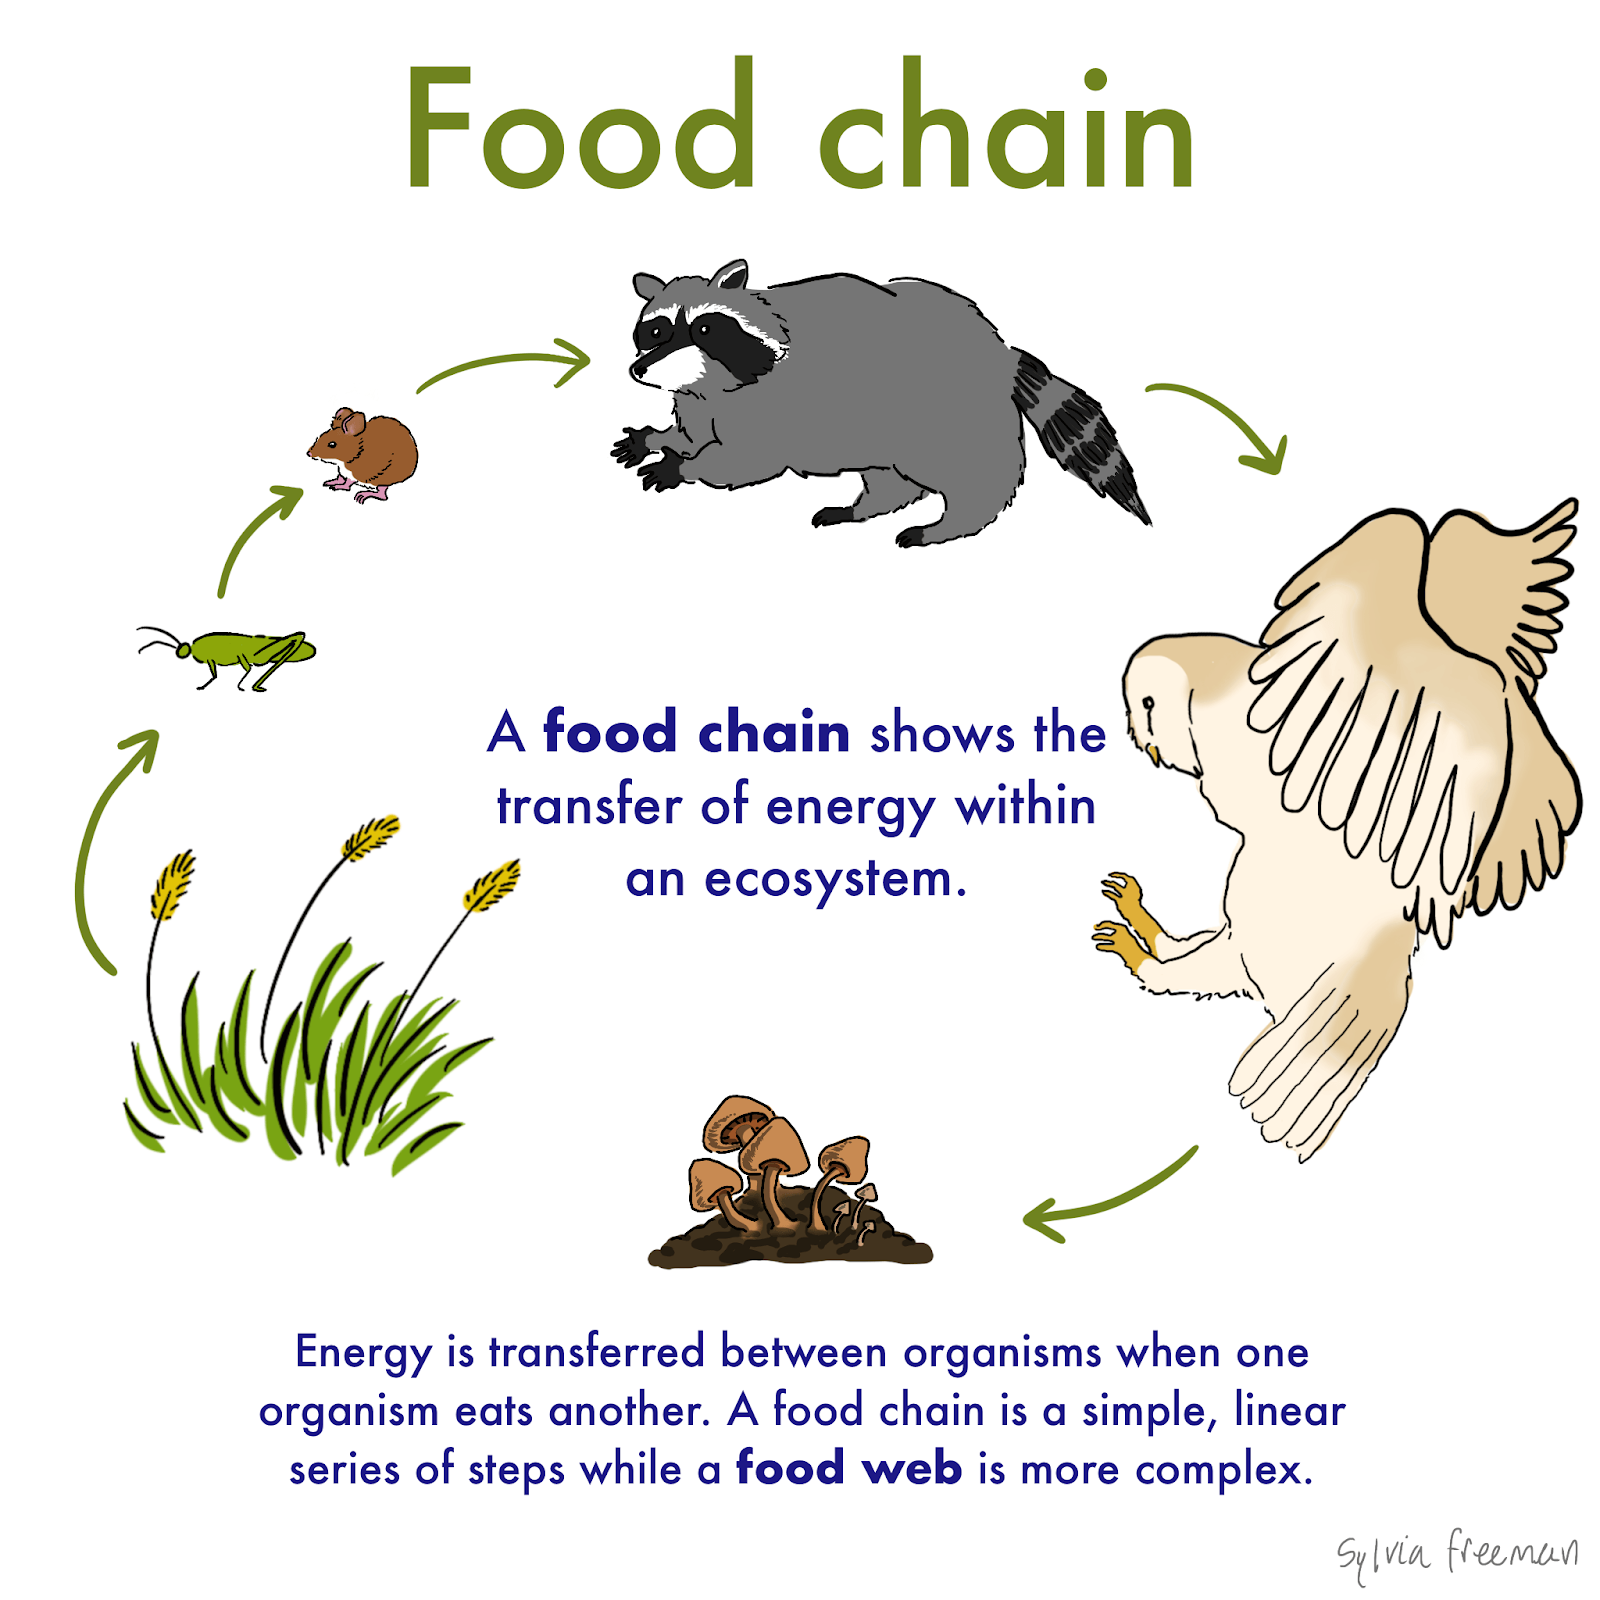
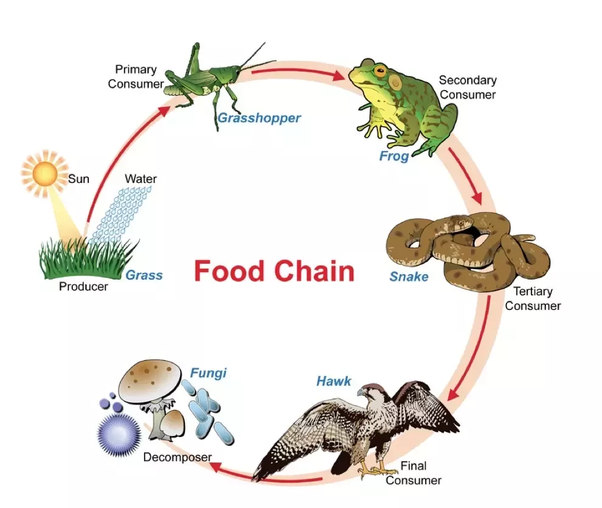
I spent three summers grading field surveys on pond ecosystems before I ever heard the term "Food Chain Definition Biology" used in a way that matched what I was actually seeing. Most textbooks treat it like a neat line from grass to deer to wolf, and that's fine for a diagram on page 47. In practice, those chains dissolve the moment you step outside with a notebook. A food chain is the linear transfer of energy and nutrients from one organism to another through feeding relationships. It starts with primary producers—plants, algae, cyanobacteria—that capture solar energy via photosynthesis. Then come herbivores that eat those producers, carnivores that eat the herbivores, and decomposers that break down dead matter at every level. Each step is a trophic level, and energy transfers between them are rough, not precise. The standard efficiency between trophic levels sits around ten percent. That means roughly ninety percent of the energy at one level is lost as heat, metabolic work, or indigestible material before it reaches the next. This is the 10% rule, and it's why food chains rarely exceed four or five links. You can't sustain a top predator if there isn't enough biomass at the bottom to feed the levels below it. Ever.
Why the Linear Model Breaks Down Immediately
Here's the part that trips up students and field researchers alike: almost no organism eats just one thing. A red-winged blackbird eats seeds, yes, but also insects. A raccoon eats frogs, berries, carrion, and roadkill. The moment you map those connections, you get a food web, not a chain. Chains are theoretical tools, not observations from the wild. I learned this the hard way during a graduate project on wetland food webs in northern Minnesota. I'd built a clean six-level chain model on paper: algae zooplankton minnow heron hawk. Then I dissected the hawks' pellets and found fish scales, vole fur, and bird bones. The hawk wasn't eating herons. It was skipping three levels entirely. My chain was wrong because it assumed a level-by-level path that doesn't reflect actual foraging behavior. The workaround was simple but humbling. I switched to stable isotope analysis—specifically carbon-13 and nitrogen-15 ratios in tissue samples—which gives you the actual dietary integration over weeks or months, not what you think an animal might eat based on proximity. Nitrogen-15 enriches with each trophic step, so you can tell whether a organism is feeding closer to the base or the top. It took me six weeks to process forty samples, but the resulting dietary maps were accurate enough to publish.
Practical Nuances Beginners Miss
One thing that doesn't get enough attention is the role of detritus. Dead organic matter—the leaves that fall into streams, the carcasses that sink to the bottom, the feces that get processed by microbes—carries more energy in most ecosystems than living plant material does. Detrital food chains often support more biomass than grazing chains, yet they're routinely omitted from textbook diagrams. In temperate forests, up to ninety percent of primary production enters the ecosystem as detritus before any herbivore touches it. Another overlooked point is omnivory. When an organism occupies more than one trophic level, it blurs the clean boxes we draw in class. Bears are classified as carnivores taxonomically, but their trophic position in a given ecosystem might sit at 2.8 on a scale where pure plants equal 2.0 and pure apex predators sit around 4.5 to 5.0. That fractional position matters for modeling energy flow accurately.
Get the Full Details
Limitations You Need to Know About
The food chain concept has real constraints. It assumes closed systems with discrete levels, which ecosystems aren't. Seasonal shifts rewire feeding relationships entirely—a frog eats insects in summer and may enter dormancy or switch prey in winter. Migration bypasses local chains altogether, with organisms importing energy from distant ecosystems through their movement. Human alteration, from fishing pressure to agricultural runoff, can collapse or redirect chains faster than models predict. If you're trying to use this framework for anything beyond classroom instruction, pair it with food web analysis or network ecology methods. Stable isotope mixing models, gut content sequencing, and bioenergetic modeling will give you results that actually match what's happening. The basic chain definition is a starting point, not a complete tool.