The Hardy-Weinberg Model as a Null Hypothesis
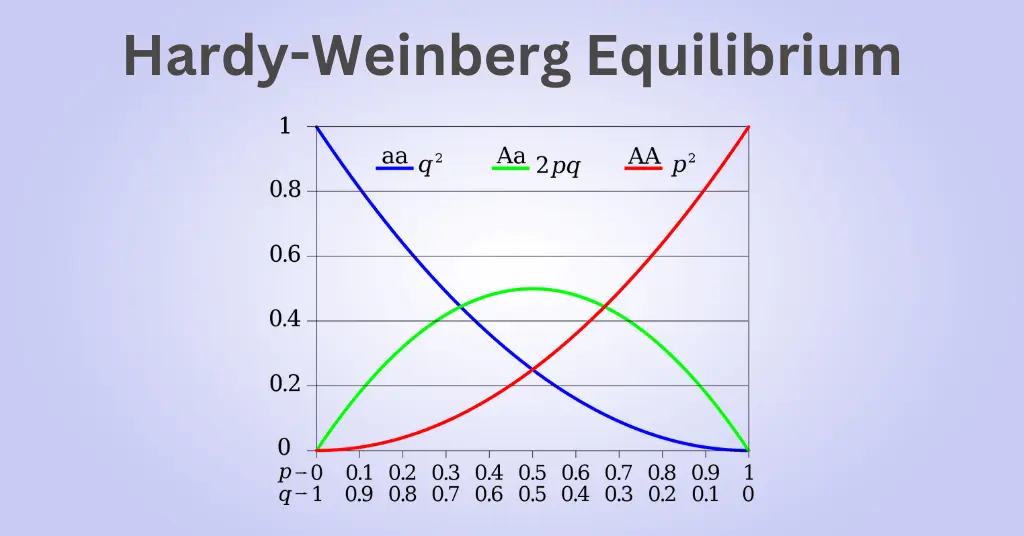
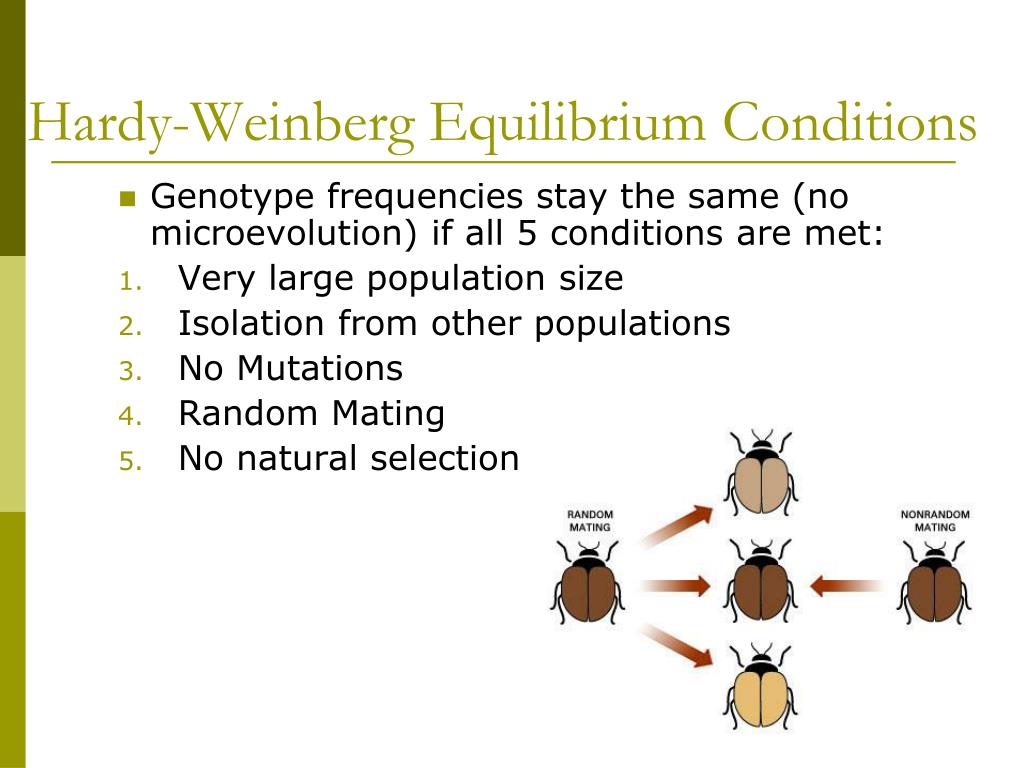
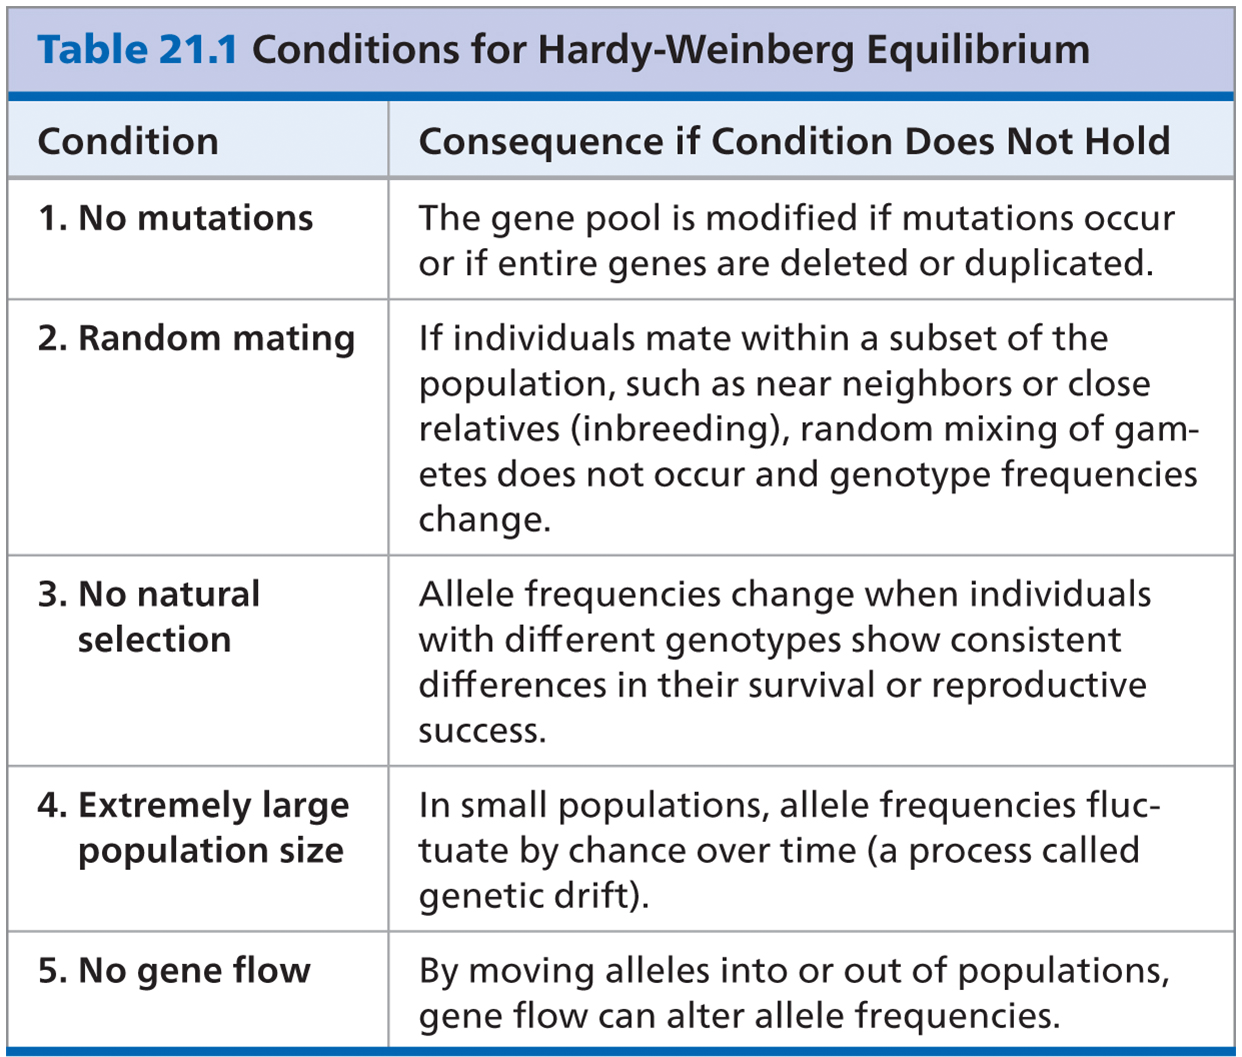
The Hardy-Weinberg Equilibrium Conditions represent five specific requirements a population must meet for allele and genotype frequencies to remain constant across generations without evolutionary change. Those conditions are no mutation, random mating, no gene flow, infinitely large population size, and no natural selection. The standard formula used is p² + 2pq + q² = 1, where p and q are allele frequencies at a single locus with two alleles. This equation gives you expected genotype frequencies if mating is random and no evolutionary force is acting on that locus. The thing most people get wrong is that Hardy-Weinberg equilibrium is not something you expect real populations to actually be in. It is a null model. You calculate what the genotype frequencies should look like under ideal conditions and then compare your observed data against that expectation. If the observed values deviate significantly, you have evidence that one or more of the five conditions is being violated. The equilibrium model itself does not tell you which condition is broken, only that something is.
Hardy Weinberg Equilibrium Conditions Explained
The five conditions work together as a single logical unit. Remove any one of them and the model's predictions no longer hold for that population. No mutation means the allele pool stays fixed unless an external source introduces new variants. Random mating means individuals pair without regard to genotype at the locus in question. No gene flow means no migrants are bringing in or taking away alleles. Infinite population size means genetic drift is mathematically negligible. No natural selection means all genotypes have equal fitness. I remember working with a conservation genetics project where a small population of a fish species showed a striking deficit of heterozygotes compared to Hardy-Weinberg expectations. The initial interpretation from the lab was inbreeding depression. I ran a microsatellite assay and the numbers looked clean on the surface, but the heterozygote deficit persisted across multiple loci. The problem turned out to be null alleles, a genotyping artifact where one allele fails to amplify during PCR, making heterozygotes appear as homozygotes. Once I accounted for null allele frequency using a correction method, the apparent deviation from equilibrium largely disappeared. Without that step, you would have attributed a technical artifact to evolutionary biology and written a very wrong conclusion. This is the kind of thing that does not make it into introductory textbooks. People memorize the five conditions, plug numbers into p² + 2pq + q² = 1, and call it done. In practice, checking whether those conditions actually hold requires more than a simple chi-squared test against expected values.
Here is the calculation approach I use when I need to assess equilibrium at a locus. First, determine the observed genotype counts from your sample. Next, calculate allele frequencies by counting alleles directly from the genotype data. Then compute expected genotype frequencies using the Hardy-Weinberg formula. Finally, run a chi-squared goodness-of-fit test comparing observed and expected counts. With a two-allele system, you have one degree of freedom after estimating allele frequency from the data. If the p-value falls below your significance threshold, the population is not in equilibrium at that locus. There is a nuance most beginners miss. Hardy-Weinberg equilibrium can be disturbed by inbreeding even when all five formal conditions are met. Inbreeding is technically a form of non-random mating with respect to genotype, but it specifically increases homozygosity without changing allele frequencies. The allele frequencies stay the same, so p and q remain valid, but the genotype frequencies shift away from p², 2pq, and q². The resulting distribution follows the inbreeding coefficient formula, where expected heterozygosity becomes 2pq(1 - F) and homozygote frequencies increase accordingly. You can detect this pattern by looking specifically at the heterozygote deficit across multiple loci. Another point people overlook is that Hardy-Weinberg equilibrium can hold even when evolutionary forces are present, as long as those forces are balanced. For example, selection against a recessive homozygote can be offset by mutation introducing new copies of that allele at the same rate. In that scenario, allele frequencies remain stable and genotype frequencies match the Hardy-Weinberg prediction, but the population is not free from evolutionary pressure. A non-significant chi-squared result does not prove the absence of evolution, only that the observable frequencies match the equilibrium expectation.
Get the Full Details

When I analyze real data, I also check for genotyping errors before invoking any biological explanation. Allelic dropout, stutter bands, and scoring mistakes can all produce patterns that mimic Wahlund effects or inbreeding. A simple way to spot this is to look at the same population across multiple loci. If every locus shows a heterozygote deficit, the cause is likely technical or population structure rather than selection at a single locus. If only one locus deviates, selection is a more plausible explanation. The Hardy Weinberg Equilibrium Conditions are still useful because they give you a baseline to work from. You can estimate carrier frequencies for recessive diseases in human populations, check whether a locus is under selection in experimental evolution studies, or identify population substructure in ecological samples. But the model has clear limitations. It assumes a single locus with two alleles, which is often not true. It does not account for linkage between loci. It treats population size as infinite, so it breaks down in small populations where drift dominates. And it cannot distinguish between different mechanisms that produce the same deviation pattern. If you need to analyze multiple loci simultaneously or work with populations that have known substructure, you are better off using methods like likelihood-based approaches or Bayesian frameworks that can incorporate uncertainty in allele frequency estimation. Software like GENEPOP or Arlequin handles exact tests for equilibrium that are more reliable than chi-squared when sample sizes are small or expected counts are low. For human medical genetics, a quick Hardy-Weinberg check is still standard practice during quality control of genome-wide association studies, but even there, the field has moved toward more sophisticated filters.
The bottom line is that Hardy-Weinberg equilibrium is a tool, not a law of nature. It tells you what should happen under a very specific set of assumptions. Real populations rarely meet those assumptions perfectly, and that is fine. The value is in measuring how far off you are and figuring out why. Use the formula correctly, validate your genotyping data first, and do not treat a non-significant result as proof that nothing interesting is happening.