Understanding Homologous Structures in Comparative Biology
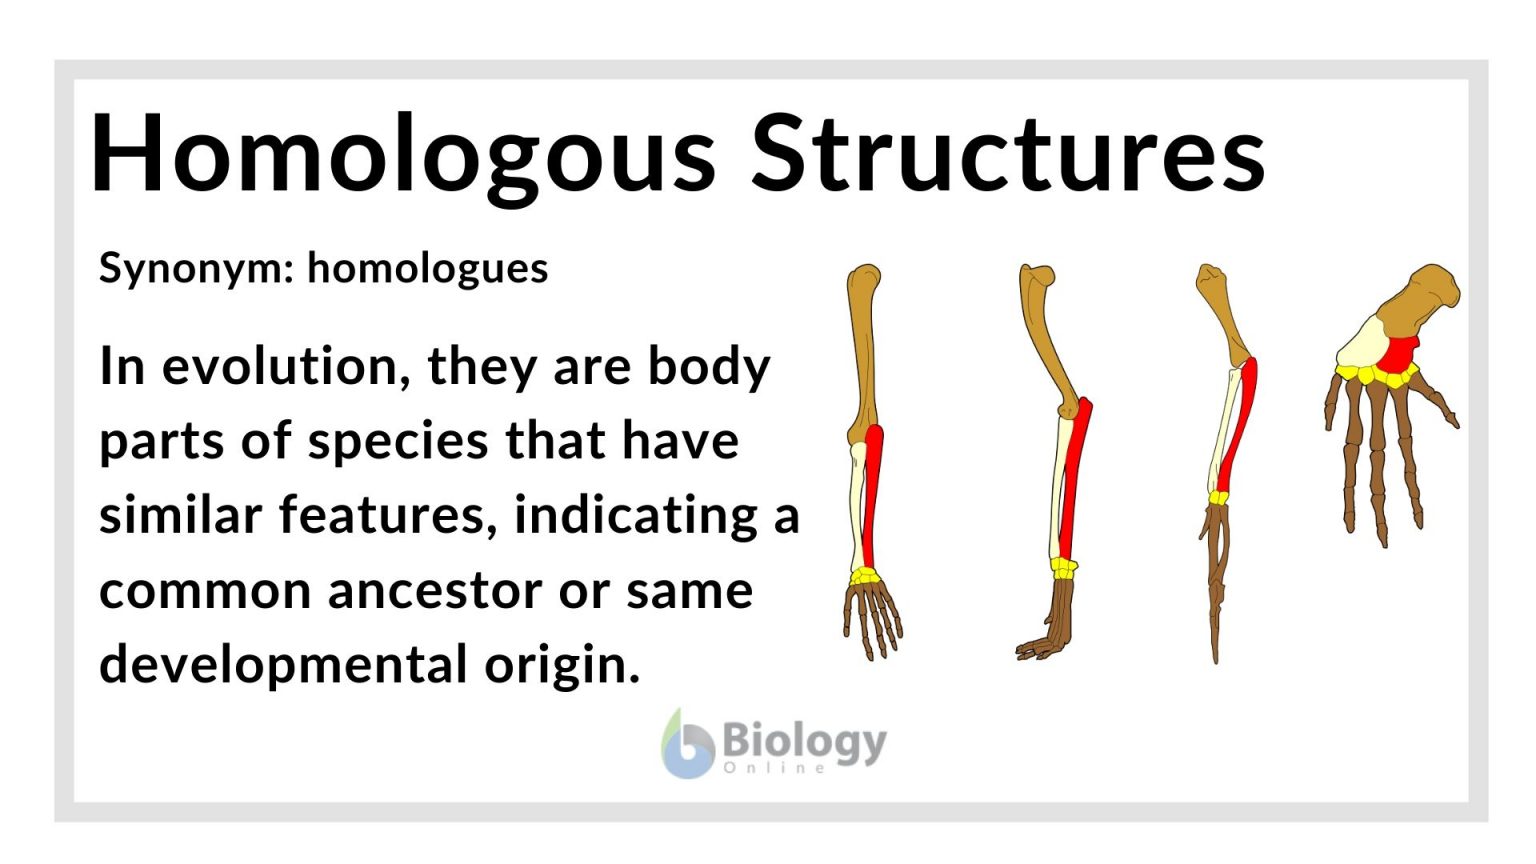
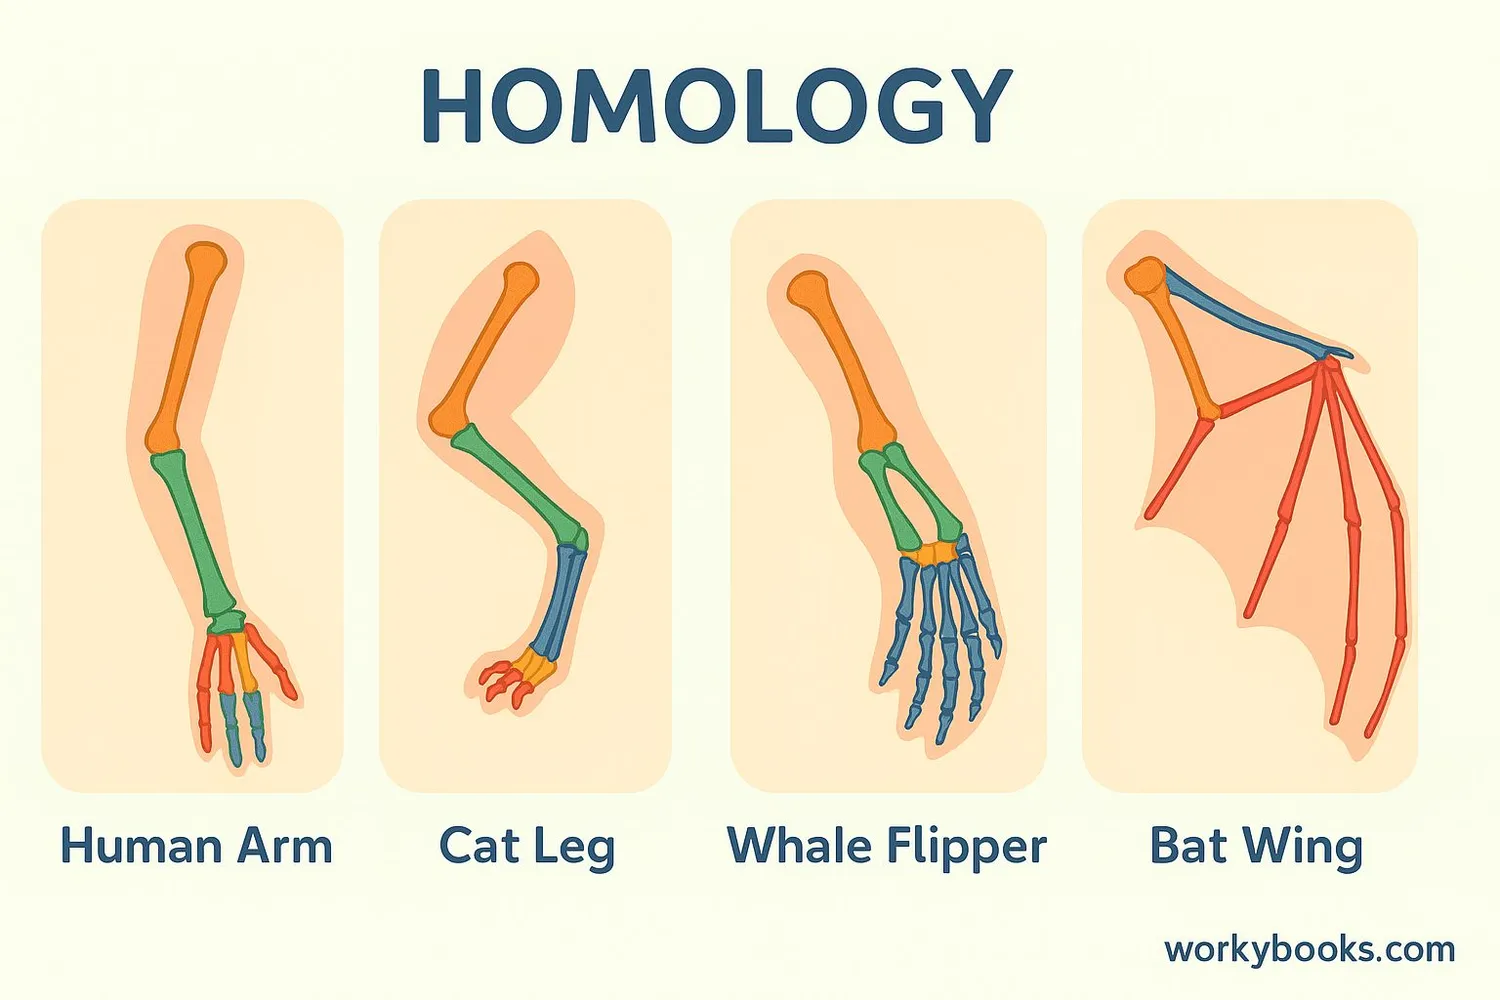
The way evolutionary biologists map structural similarity across species usually starts with the forelimbs of tetrapods. You look at a human hand, a bat wing, a whale flipper, and a horse leg and you see the same underlying bone layout: one large bone, two smaller forearm bones, a cluster of wrist elements, and digit rays. That common blueprint inherited from a shared ancestor is what the homologous structures definition biology framework is built around. It is one of the most straightforward concepts in evolutionary morphology, but it gets misapplied constantly in introductory courses and even in some exam questions. Homologous structures are anatomical features found in different species that share a common evolutionary origin, regardless of whether they currently perform similar functions. The key word is origin, not function. A bird wing and a bat wing are homologous as forelimbs because both descend from the same ancestral tetrapod limb structure. They are analogous as flying surfaces because flight evolved independently in each lineage. Confusing those two categories is the most common error I see when grading undergraduate work. In practice, establishing homology requires more than a visual comparison. You need to trace developmental pathways, examine embryonic origin, and compare underlying skeletal or muscular architecture. Two structures can look alike on the outside and still not be homologous if they arise from different developmental programs. Convergent evolution produces that kind of surface similarity regularly, especially in marine organisms and desert-dwelling species.
I spent several years working on morphological datasets for vertebrate phylogenetics, and one edge case still comes to mind. We were comparing the jaw suspension mechanisms in certain species of salamanders, specifically how the quadrate bone articulates with the skull. On paper, the structures looked homologous across the taxa we were studying. The bone positions matched, the general shape was consistent, and the literature supported homology assignments. But when we ran the phylogenetic analysis, the salamander clade kept grouping with outgroups in ways that made no anatomical sense. The problem turned out to be secondary loss. Some species had secondarily reduced the quadrate to near non-function, and the remaining remnant structure had been misidentified as homologous when it was actually a degraded descendant that no longer carried the full diagnostic features. We ended up re-examining the embryonic development of that bone in the affected species and realized the homology signal was still there, just buried under significant modification. It took about three weeks of fresh dissections and micro-CT scanning to sort it out. The workaround was to weight the homology character differently in the matrix, giving more importance to developmental origin data than to adult morphological appearance alone.
How Homology Gets Determined in Practice
The standard approach involves multiple lines of evidence stacked together. Morphological comparison forms the foundation, but it is never sufficient on its own anymore. Developmental biology provides the next layer, looking at which germ layers contribute to the structure and how the pattern forms during ontogeny. Molecular data adds a third dimension, with gene expression patterns like Hox gene domains serving as powerful confirmatory tools. When all three lines agree, you have a robust homology claim. When they disagree, you have a research problem. One thing beginners consistently miss is that homology exists at multiple levels of organization. A bone can be homologous at the organ level but not at the tissue level. A muscle can be homologous in attachment but not in fiber orientation. A gene regulatory pathway can be homologous while the endpoint structure it produces looks completely different. You need to specify which level you are talking about, and most people do not bother. Another counter-intuitive point is that highly modified structures can be more useful for establishing deep homologies than conserved ones. When a structure stays roughly the same across millions of years, it is harder to tell whether similarity reflects shared ancestry or simply functional constraint. A structure that has been radically reshaped by evolution, like the mammalian middle ear bones derived from jaw elements, actually provides stronger evidence for common descent because the functional repurposing makes independent evolution far less plausible.
Get the Full Details
Common Pitfalls and Where the Framework Breaks Down
The biggest limitation of homology-based reasoning is that it becomes unreliable when dealing with organisms that have extremely reduced or highly derived body plans. Parasitic organisms, for example, often lose structures entirely or reduce them to vestiges that are nearly impossible to align across species. In those cases, molecular phylogenetics usually replaces morphological homology assessment as the primary tool, and even then the results can be ambiguous. Another hard boundary is radial symmetry and body plans that do not share the segmental organization of bilaterians. Comparing a jellyfish tentacle to an arthropod appendage using classical homology frameworks does not work productively. You need entirely different analytical approaches for those groups, and trying to force homology language onto them tends to produce meaningless results. There is also the problem of serial homology, where repeated structures within a single organism, like vertebrae or insect body segments, complicate cross-species comparisons. Are two adjacent vertebrae homologous to each other within one individual, and how does that relationship map onto vertebral homology across different species? The answer depends on whether you treat serial repeats as copies of a developmental module or as independently generated elements, and different researchers draw that line differently.
Practical Workflow for Identifying Homologous Structures
If you are working through a comparative anatomy problem, start by documenting the structure in as much detail as possible before making any homology claims. Take measurements, note attachment points, trace the nerve and blood supply if accessible, and photograph everything from multiple angles. Visual memory is unreliable for this kind of work. Next, consult the developmental literature for the species in question. Even a brief look at embryonic staging papers can reveal whether two structures share an origin or arose independently. This step typically takes 20 to 40 minutes depending on how well-documented the species is, and it prevents a lot of downstream errors. Then build a character matrix if you are doing phylogenetic work. Code presence or absence, note transformation series where applicable, and mark uncertain homologies as missing data rather than forcing a decision. Rushing to code ambiguous structures as definite homologies is how bad trees get built, and correcting those mistakes later usually takes three to five times longer than doing it right the first time.
Finally, test your homology assumptions against alternative hypotheses. Run the analysis with and without the questionable characters, check whether key clades remain stable, and be willing to revise your codes when the data contradicts your initial assumptions. The goal is not to prove your homology claims correct, it is to find out whether they hold up under scrutiny.


