Understanding Cellular Energy Harvesting
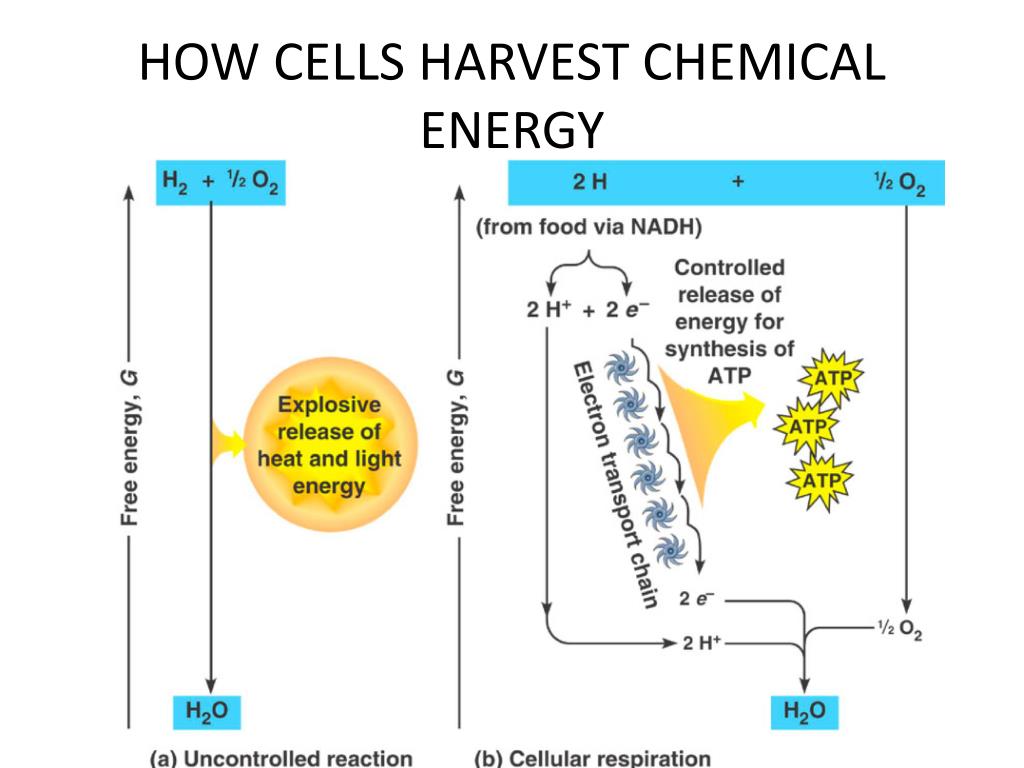
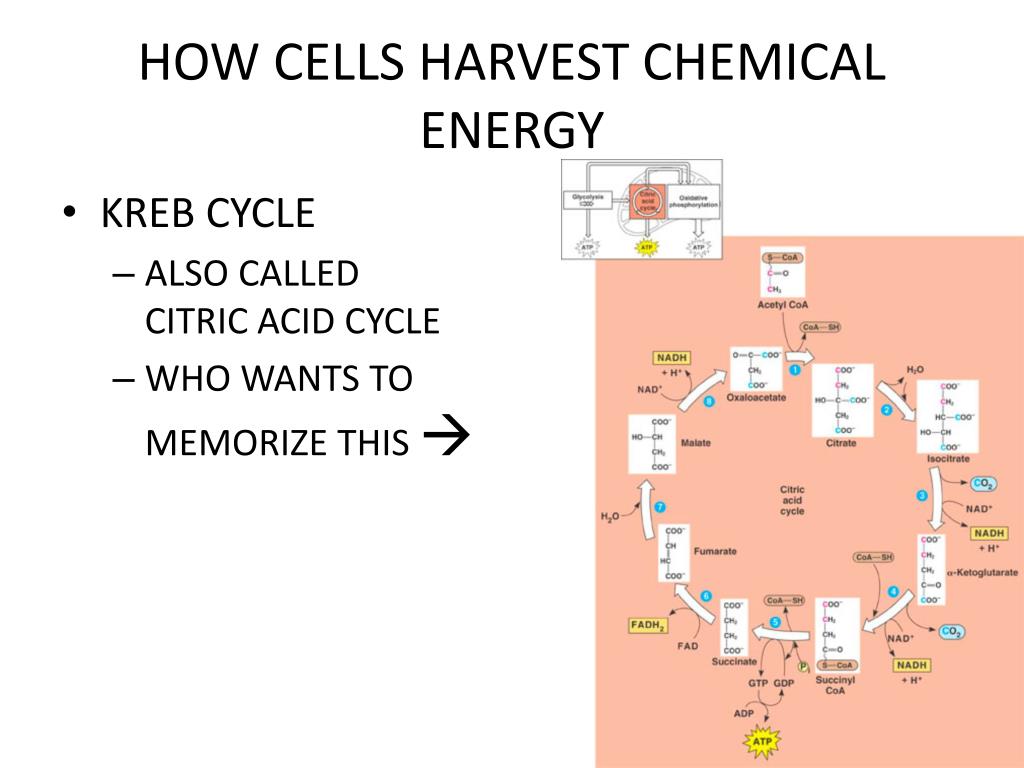
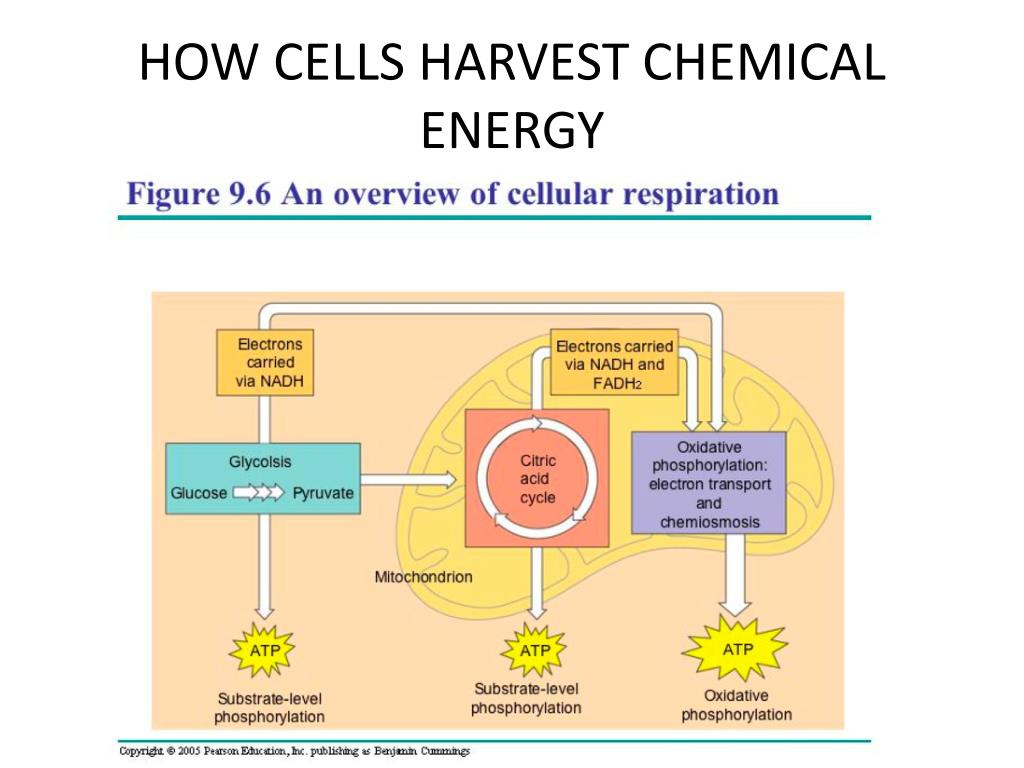
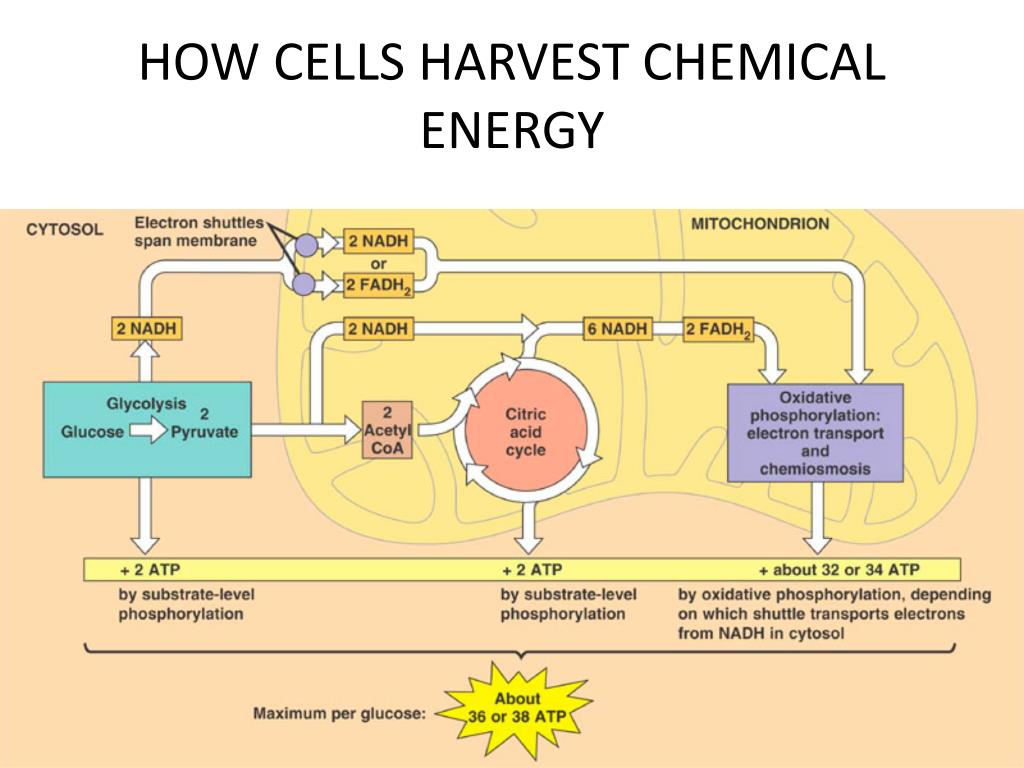
Cells break down glucose and other fuel molecules through a series of enzyme-catalyzed reactions that transfer electrons to carriers like NAD+ and FAD. The energy released during these transfers gets stored temporarily as a proton gradient across a membrane, and that gradient drives ATP synthase to produce the actual currency cells spend. Most textbooks present this as glycolysis, the Krebs cycle, and oxidative phosphorylation, but the reality is messier than that. I spent a lot of time working with isolated mitochondria in grad school, and the first thing I learned was that nothing works in isolation. You cannot understand glycolysis without understanding why it even happens where it happens. Glycolysis runs in the cytoplasm because that is where the enzymes are. It does not require oxygen. It produces a net gain of two ATP and two NADH per glucose molecule. That is the baseline. From there, things get more complicated depending on whether oxygen is available. When oxygen is present, pyruvate enters the mitochondrion. The pyruvate dehydrogenase complex converts it to acetyl-CoA, releasing one CO2 and reducing one NAD+. That acetyl group then feeds into the citric acid cycle. The cycle turns once per acetyl-CoA, producing three NADH, one FADH2, one GTP (which gets converted to ATP), and two more CO2 molecules. Per glucose molecule, that is double because you start with two pyruvates. The yield numbers are what you will see on every exam, but the actual stoichiometry in a living cell is somewhat different because of proton leak and transport costs.
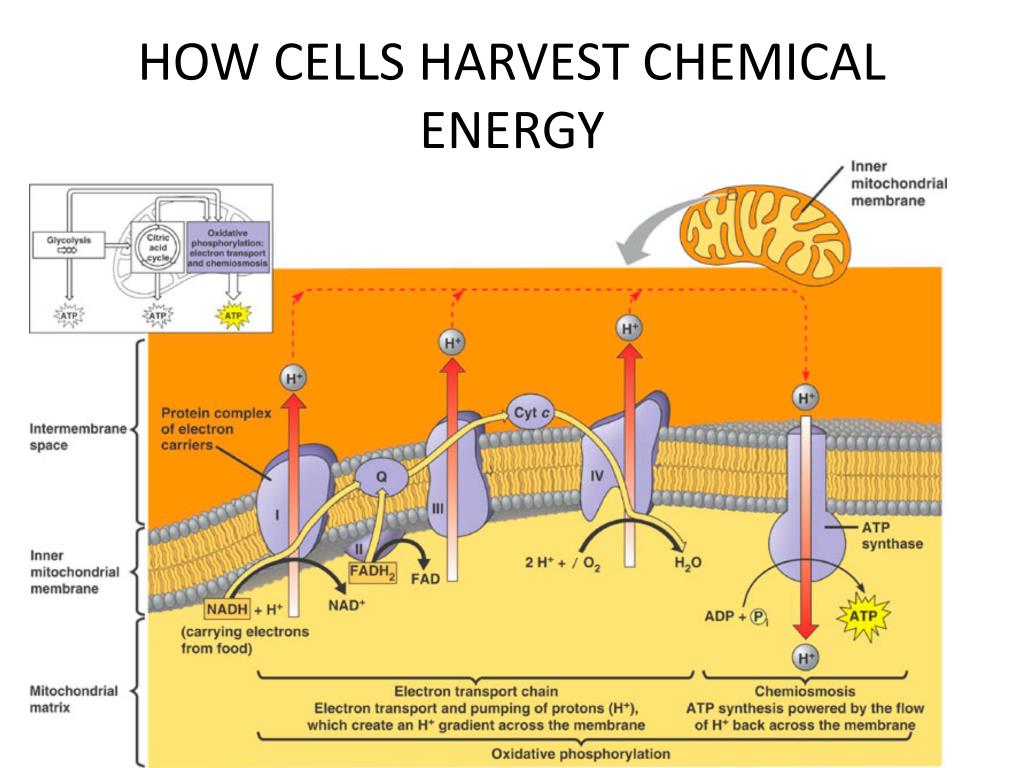
The electron transport chain is where people typically get confused. The four protein complexes do not sit next to each other in a neat line. They exist as supercomplexes in some tissues, and ubiquinone and cytochrome c shuttle electrons between them. Each NADH that enters at Complex I can theoretically drive the pumping of enough protons to make about 2.5 ATP. Each FADH2 entering at Complex II bypasses the first pumping site and yields roughly 1.5 ATP. These are theoretical maximums. The P-O ratio varies by cell type, membrane potential, and even the growth conditions of the organism. One thing nobody tells you upfront is that the proton gradient is not just for ATP production. It also drives the import of phosphate, pyruvate, and ADP/ATP exchange through the inner mitochondrial membrane. If that gradient collapses for any reason, transport stops, and the cell starves even if glucose is flooding in. I remember running an experiment where I added a low dose of FCCP, a protonophore, and watched the ATP output drop to near zero while oxygen consumption spiked. The mitochondria were burning fuel faster but producing nothing usable. That is uncoupling, and it happens physiologically in brown adipose tissue for thermogenesis. It also happens pathologically in sepsis and mitochondrial toxins. Glycolysis itself has regulatory checkpoints worth paying attention to. Phosphofructokinase-1 is the main one. It is inhibited by high ATP and citrate and activated by AMP and fructose-2,6-bisphosphate. That last molecule is controlled by PFK-2, which is itself regulated by phosphorylation through hormonal signaling. In the liver, glucagon triggers a cascade that lowers fructose-2,6-bisphosphate and slows glycolysis. Insulin does the opposite. This is not just academic. It explains why your liver stops making glucose during a fed state and why exercise suddenly ramps up glycolytic flux in muscle.
The Cori cycle is another piece that gets glossed over. Muscle cells running anaerobic glycolysis produce lactate. That lactate travels to the liver, gets converted back to pyruvate, then to glucose via gluconeogenesis, and returns to the muscle. The cycle costs six ATP equivalents but allows glycolysis to keep running when oxygen is limiting. It is inefficient in isolation but essential during sustained exercise or in tissues that cannot rely on constant oxygen supply. The brain does not use this pathway effectively, which is why lactic acidosis from prolonged seizures is so dangerous. There is a common misconception that the Krebs cycle is just a linear pathway. It is actually amphibolic, meaning it serves both catabolic and anabolic functions. Intermediates siphon off for amino acid synthesis, heme production, and gluconeogenesis. When those intermediates are drained, the cycle slows unless there is anaplerotic input. Pyruvate carboxylase replenishes oxaloacetate from pyruvate. This is critical in tissues with high biosynthetic demand, like rapidly dividing cells. Cancer cells exploit this by upregulating pyruvate carboxylase and running the cycle in a branched, not purely cyclic, manner. That is why targeting cycle intermediates is a real therapeutic strategy. If you want to measure how efficiently a cell harvests energy, the standard approach is Seahorse analysis or similar extracellular flux measurement. You inject oligomycin to block ATP synthase and measure the proton leak component. Then you inject FCCP to maximize electron transport and find the spare respiratory capacity. Rotenone and antimycin A shut down the chain entirely to get non-mitochondrial respiration. The data gives you basal respiration, ATP-linked respiration, proton leak, maximal respiration, and spare capacity. Those five numbers tell you more about mitochondrial health than any single ATP count ever could.
Get the Full Details
One edge case that bit me more than once: when working with primary cells rather than cell lines, the oxygen consumption rate can vary wildly between passages and even between wells on the same plate. I wasted two weeks trying to normalize data before realizing that the seeding density was inconsistent because the cells adhered at different rates. The fix was switching to a colorimetric protein assay for normalization instead of relying on cell count or total DNA. Small thing, made a huge difference. Fermentation is what cells fall back on when the electron transport chain is not operational. Yeast converts pyruvate to ethanol and CO2. Muscle cells convert it to lactate. Both regenerate NAD+ so glycolysis can continue. The ATP yield is two per glucose either way. The difference between fermentation and anaerobic respiration is that the latter uses an electron transport chain with a final acceptor other than oxygen, like sulfate or nitrate. Some bacteria do this. Human cells do not. If you see someone conflate fermentation with anaerobic respiration, they do not actually know the difference. Shewanella and Geobacter species use outer membrane cytochromes to transfer electrons to insoluble Fe3+ minerals. That is extracellular electron transfer, and it has implications for bioelectronics and bioremediation. But that is microbial. For eukaryotic cells, the story ends at the inner mitochondrial membrane and the ATP synthase rotor. The mechanism is rotation catalysis. Protons flow through the FO subunit, the c-ring spins, the gamma subunit rotates inside the beta subunits of the F1 head, and each 120-degree turn synthesizes one ATP. Three protons pass through for each turnover, plus one more for the phosphate translocase. The exact H+/ATP ratio depends on the number of c-subunits in the ring, which varies between species. Humans have eight, some organisms have fifteen. That single structural difference changes the energy yield per glucose significantly.
Regulation is layered across all three stages. Glycolysis responds to energy charge through PFK-1 and pyruvate kinase. The link reaction is controlled by the NADH/NAD+ ratio and acetyl-CoA accumulation. The citric acid cycle responds to ADP availability, NADH, and ATP. Oxidative phosphorylation is controlled almost entirely by ADP concentration, which is why it is called respiratory control. Add ADP, the chain speeds up. Run out of ADP, it slows down. It is that simple in principle, though the kinetics involve allosteric modulation, post-translational modifications, and gene expression changes over longer timescales. One pitfall beginners run into is assuming that more electron transport always means more ATP. It does not, because proton leak and uncoupling proteins dissipate the gradient as heat. UCP1 in brown fat is intentional. UCP2 and UCP3 are expressed more broadly and may protect against oxidative damage by lowering the proton motive force slightly. Under pathological conditions, uncoupling becomes excessive and contributes to wasting syndromes. Measuring the uncoupling proteins' activity requires separating oligomycin-resistant respiration from true leak, which is easy to botch if you are not careful with your inhibitors and controls. The efficiency of aerobic respiration is often quoted as around forty percent. That means forty percent of the free energy from glucose oxidation gets captured in ATP, and the rest is lost as heat. The remaining sixty percent is not wasted in a biological sense. Heat maintenance is vital for endotherms. But from a pure energy conversion standpoint, it is a loss. No engine in a car runs at forty percent efficiency either. Diesel engines top out around fifty-five percent. Biology is not trying to be efficient in an engineering sense. It is trying to be functional under fluctuating conditions with self-repairing components made of water-soluble proteins.
If you are studying this for an exam, focus on the regulatory steps and the stoichiometry. If you are actually working in a lab, focus on the assumptions behind every number you calculate. The theoretical yield of thirty-six or thirty-eight ATP per glucose is wrong in almost every real system. The actual yield is closer to thirty ATP, and it varies by cell type, metabolic state, and membrane integrity. The difference matters when you are modeling metabolism or interpreting flux data.