The Basic Mechanics of Prokaryotic Cell Division
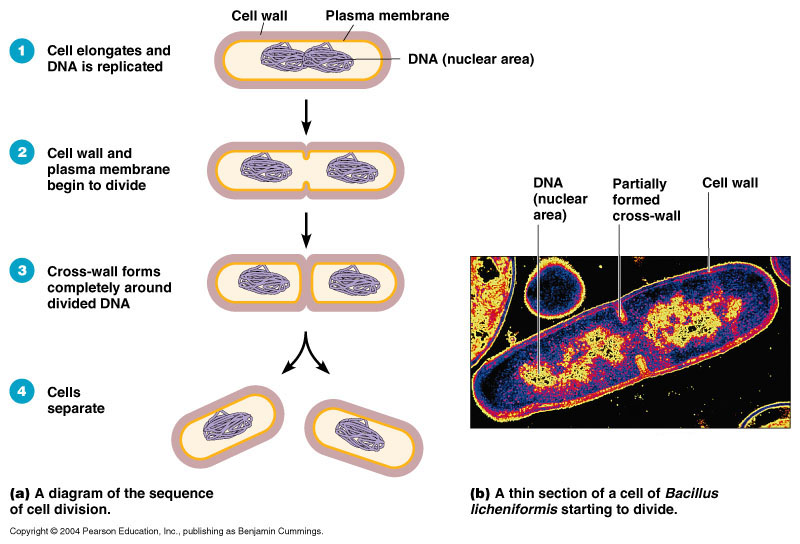
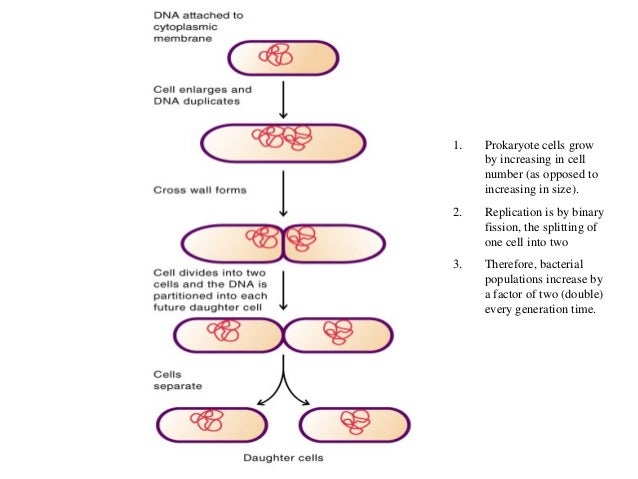
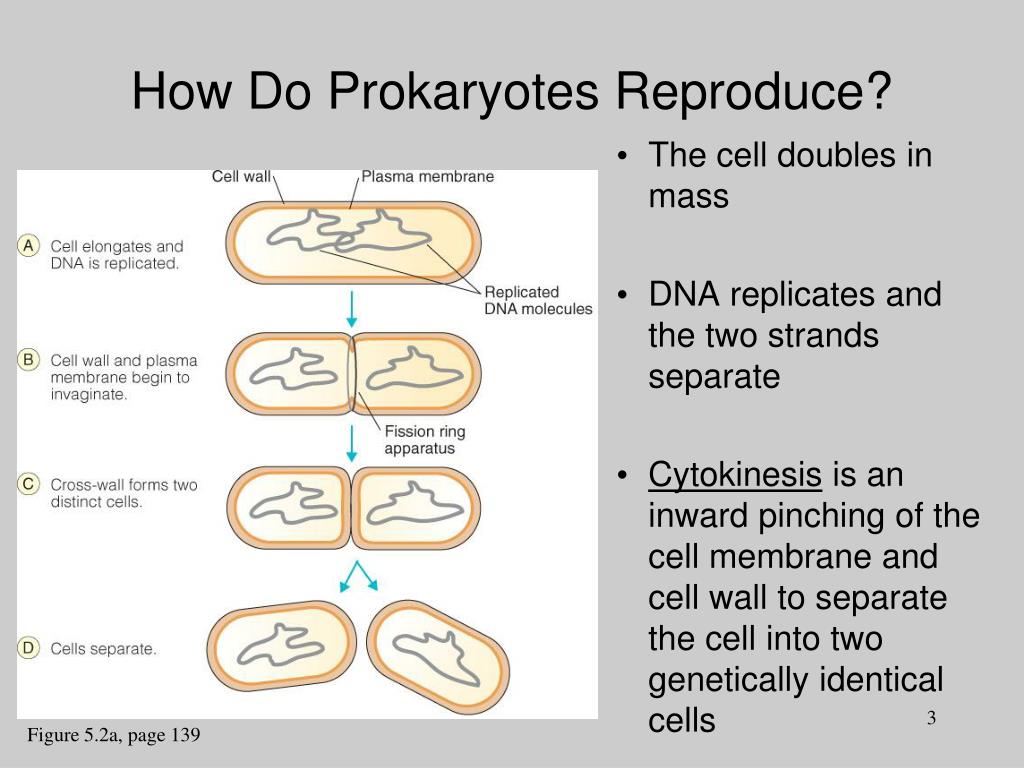
Prokaryotes reproduce through a process called binary fission. It is not complicated, but it is easy to misunderstand if you have only ever read a textbook diagram. The cell replicates its single circular chromosome, then elongates, and splits into two roughly equal daughter cells. That is the short version. The actual process involves coordinated steps involving the FtsZ protein ring, DNA segregation machinery, and cell wall synthesis enzymes working in a specific temporal sequence. When I first started working with bacterial cultures in a lab setting, I assumed binary fission was just a clean split like the textbook drawings showed. It is not. Cells can and do show variation in size between daughter cells, sometimes significant variation. Chromosome segregation is not perfectly symmetrical either. The thing that matters most is the timing of Z-ring formation relative to nucleoid occlusion, which prevents the division septum from forming over unsegregated DNA.
How Do Prokaryotes Reproduce
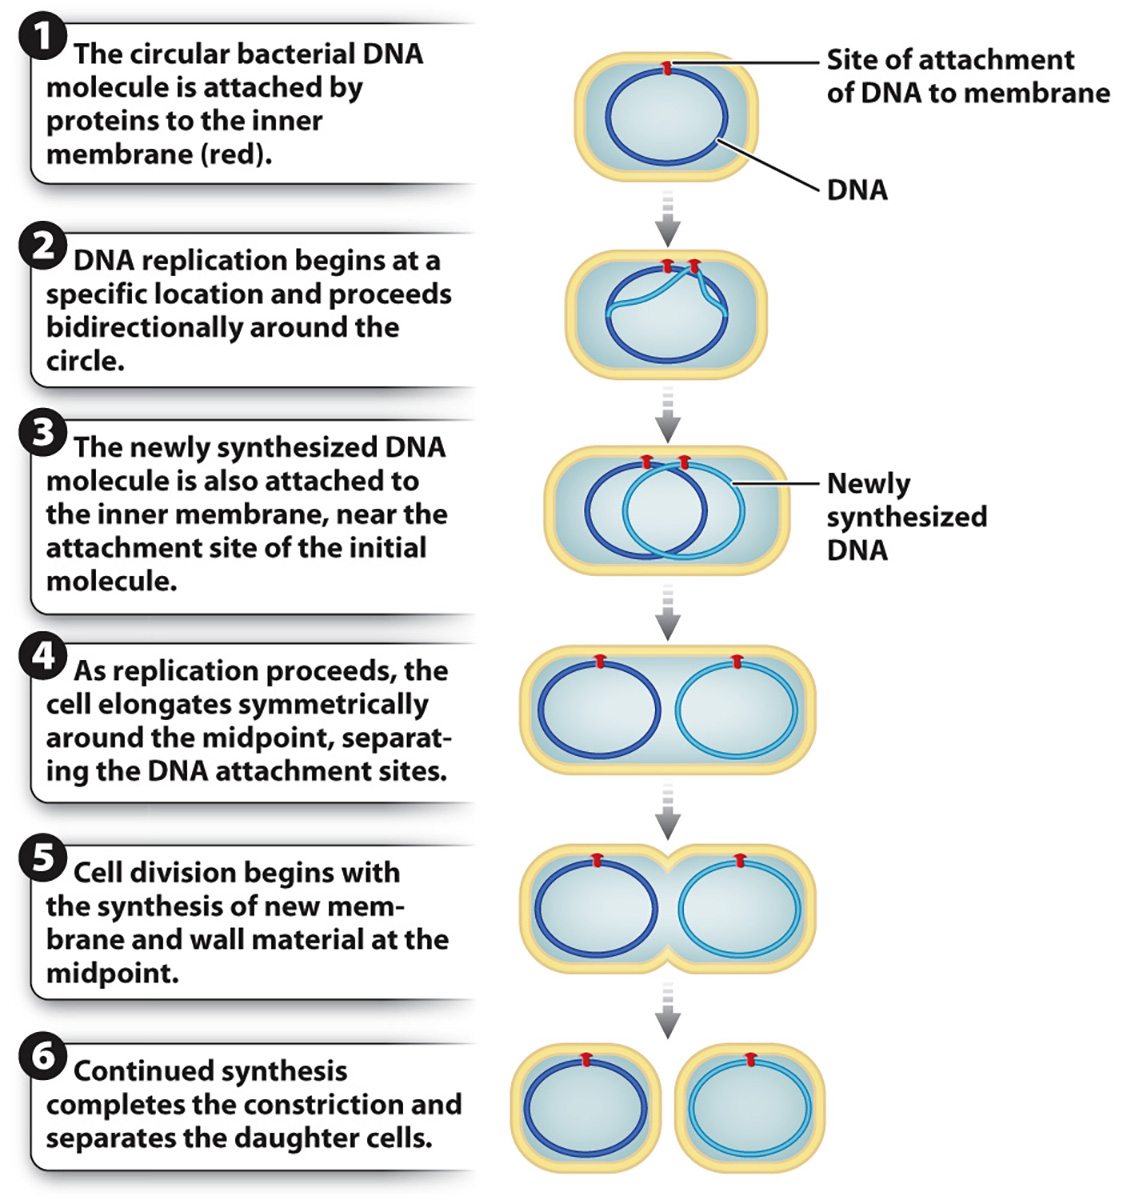
The chromosome exists as a single circular DNA molecule attached to the cell membrane at a region called the origin of replication. Replication begins at that origin and proceeds bidirectionally around the circle until the two replication forks meet at the terminus region. Once replication is complete, the two copies of the chromosome are actively moved toward opposite poles of the cell. This segregation is driven by a combination of cytoskeletal proteins like ParM in some species and the physical constraints of the growing cell envelope. After the chromosomes have moved apart, a protein called FtsZ assembles into a ring at the future division site, roughly mid-cell. FtsZ is a tubulin homolog. It polymerizes into filaments that constrict over time, drawing the cell membrane and cell wall inward. Other proteins join the ring including FtsA, ZipA, FtsK, FtsQ, FtsI, and FtsN in the standard order. Each one has a specific role in septal peptidoglycan synthesis and membrane invagination. The septum builds inward from the cell periphery until the two daughter cells are physically separated. In some species a final cleavage step mediated by autolysins completes the division. In others the daughters remain attached for a period, forming chains or clusters depending on the plane of division.
I ran into a problem once where my E. coli cultures were producing microcolomies instead of discrete colonies on agar plates. The issue was not contamination or growth medium. The cells were undergoing incomplete cytokinesis due to a temperature-sensitive mutation in the FtsA protein that had crept into the culture during repeated passaging. Switching to freshly streaked stocks from a 80°C freezer and growing at 30°C instead of 37°C resolved it immediately. The FtsA mutation only became problematic at the higher temperature.
Get the Full Details
Exceptions and Alternative Reproductive Strategies
Binary fission is the dominant mode, but it is not universal across all prokaryotes. Some bacteria reproduce through budding, where a smaller daughter cell pinches off from a larger parent. Candidatus Magnetobacterium bavaricum and Hyphomicrobium species do this. The bud starts as a small outgrowth, replicates a chromosome, and separates after reaching a certain size. It is slower than binary fission and produces asymmetric cells, which matters for things like surface attachment and motility. Cyanobacteria present another variation. Many divide through multiple fission, where the cell undergoes several rounds of chromosome replication without immediate cytokinesis, creating a multinucleoid cell before splitting into many daughter cells at once. Some species form specialized structures called akinetes, which are thick-walled resting cells that do not divide until conditions improve. They are not a reproductive strategy per se but they function similarly in population maintenance. Then there is the whole issue of plasmid distribution. Plasmids are extrachromosomal DNA elements that replicate independently of the chromosome. They use their own origins of replication and partition systems. If a plasmid lacks an active partition mechanism, segregation becomes random. I have seen cultures lose high-copy-number plasmids within a few generations simply because the selective pressure was removed and the plasmid imposed a metabolic burden. The workaround was always to maintain continuous antibiotic selection or to re-engineer the plasmid with a stable partition system like the parABS operon.
Growth Rates and What Actually Controls Them
Under ideal laboratory conditions, E. coli can double every 20 minutes. That number gets cited constantly but it is misleading without context. The 20-minute generation time assumes rich medium like LB or M9 with glucose, optimal temperature, proper aeration, and a low inoculum density. In natural environments, doubling times are measured in hours or days, sometimes longer. Nutrient limitation, temperature shifts, osmotic stress, and competition from other microbes all slow replication significantly. The speed of reproduction is ultimately constrained by the availability of building blocks. A single E. coli cell contains approximately 4 million base pairs of DNA and requires thousands of proteins, lipids, and peptidoglycan precursors to divide. Rapid division means the cell must synthesize all of that in parallel. Ribosome content scales with growth rate. Fast-growing cells can contain up to 70,000 ribosomes. Slow-growing cells have fewer than 2,000. The cell regulates this through the stringent response, which shuts down ribosomal RNA transcription when amino acid availability drops. Another constraint people overlook is the relationship between replication and division timing. In fast-growing E. coli, a new round of chromosome replication can begin before the previous round finishes. The chromosome has multiple replication forks active simultaneously. This means the cell division cycle and the DNA replication cycle are loosely coupled. A mutation that disrupts this coordination, such as one affecting the DnaA protein or the nucleoid occlusion system, can cause lethal outcomes like guillotining the chromosome during septum closure.
Common Misconceptions About Prokaryotic Reproduction
The biggest misconception is that prokaryotic reproduction is cloning. Binary fission produces genetically identical daughters under normal conditions, yes, but mutations occur during every round of replication. E. coli has a mutation rate of approximately one error per 10^9 base pairs copied. That means each division introduces roughly four to five new mutations into each daughter genome. Over many generations this adds up and is the primary source of genetic variation in asexual populations. Another misconception involves the idea that prokaryotes have no sexual reproduction. They do not reproduce sexually in the eukaryotic sense, but they do exchange genetic material through conjugation, transformation, and transduction. These are not reproductive processes because they do not increase cell number. They are horizontal gene transfer mechanisms that introduce genetic variation into populations. Confusing HGT with reproduction is a common mistake in introductory courses and it matters because the two processes operate on different timescales and have different evolutionary implications. Conjugation requires direct cell-to-cell contact through a pilus. Transformation involves uptake of free DNA from the environment. Transduction uses bacteriophages as vectors. None of these produce new cells. They modify the genetic content of existing cells. The cells still divide by binary fission or one of its variants afterward.
Practical Considerations for Working with Dividing Prokaryotes
If you are growing prokaryotes in a lab, the things that matter most are inoculum density, medium composition, and oxygen availability for aerobic species. Starting a culture from an overnight stock at too high a density can cause problems. The cells enter stationary phase artifacts and the lag phase disappears or shortens unnaturally, which skews growth curve data. The standard practice is a 1:100 dilution into fresh medium, but even that is not universal. Some slow-growing species need 1:1000 or lower. Aeration is critical for aerobic bacteria. A 50 mL culture in a 250 mL flask with 10 mL of medium shaken at 250 rpm will grow differently than the same culture in a tight-cap tube. Oxygen transfer rate limits growth rate more than nutrient availability in many standard lab setups. If your cultures are consistently slower than expected, check the shaking speed and flask fill ratio before adjusting temperature or medium recipes. Antibiotic selection adds another variable. Antibiotics that target cell wall synthesis like ampicillin do not kill dividing cells immediately. They prevent septum formation, causing cells to elongate into filaments. Filamentation is often misinterpreted as growth arrest when it is actually division inhibition. If you are using ampicillin for plasmid selection and notice filamentous cells, the plasmid is being maintained but the cells are under significant stress. Carbapenem-based antibiotics like carbenicillin are gentler alternatives that reduce filamentation while maintaining selection pressure.
The storage method also affects observed reproduction rates upon revival. Viable counts drop during frozen storage even at 80°C. Ice crystal formation causes sublethal damage to cell membranes. Thawing on ice rather than at 37°C reduces further membrane stress. A typical competent cell preparation thawed and plated will show 10^8 to 10^9 CFU/mL after overnight growth, but the actual survival rate from freeze to outgrowth is usually around 60 to 80 percent depending on the strain and storage conditions.