What Actually Drives Genetic Diversity Up
Increased Genetic Diversity Is A Result Of
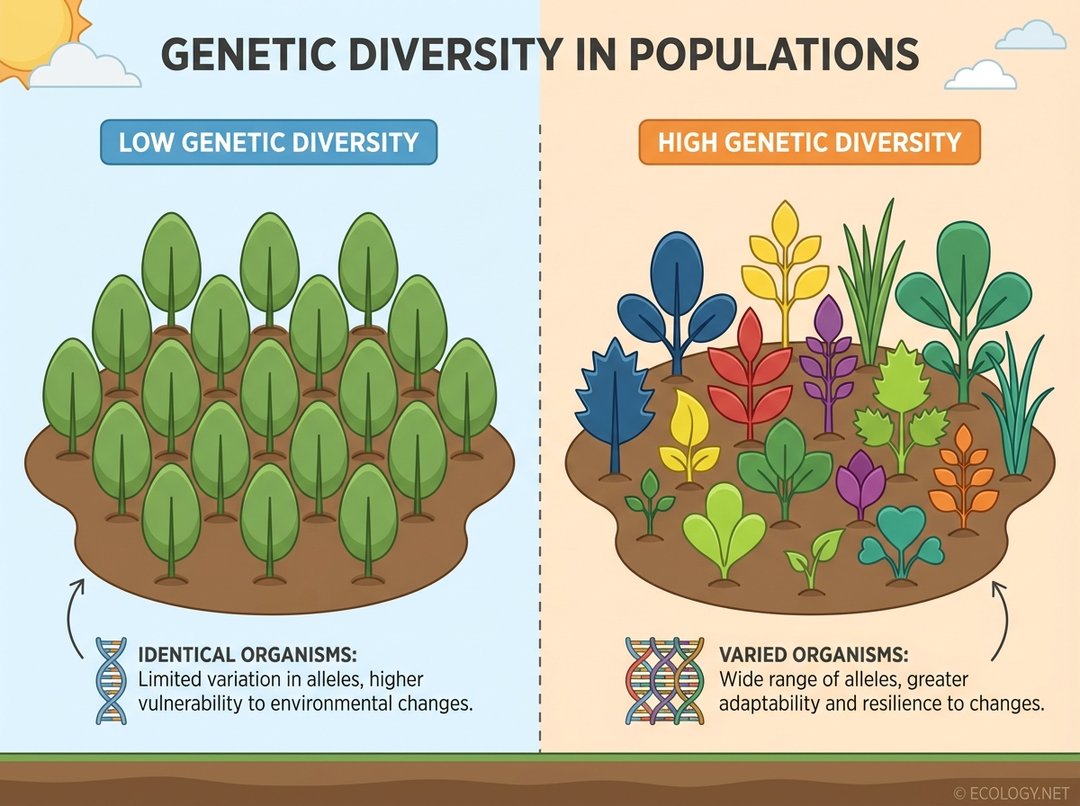
Mutation, recombination, and gene flow. That's the short version. But in practice, anyone who's actually worked with populations knows it's never just one of those things operating in isolation. You'll see a population bounce back genetically after a bottleneck, but if you don't understand which mechanism did the heavy lifting, you're going to mismanage the next one. I spent years looking at breeding programs for endangered species, and the most common mistake I see people make is assuming that simply increasing population size will restore diversity. It doesn't, not fast enough on its own. I once had a facility where they'd imported what they thought was a diverse stock of animals for a reintroduction program. The problem was those "diverse" individuals came from three different zoos but all traced back to a single founder population from forty years prior. The genetic tests looked fine at first glance, but the effective population size was roughly a quarter of the head count. We ended up having to phase out the most overrepresented lines and bring in fresh stock from an entirely separate geographic subspecies, which is a move that sounds extreme until you see the marker data.
The Three Mechanisms And How They Interact
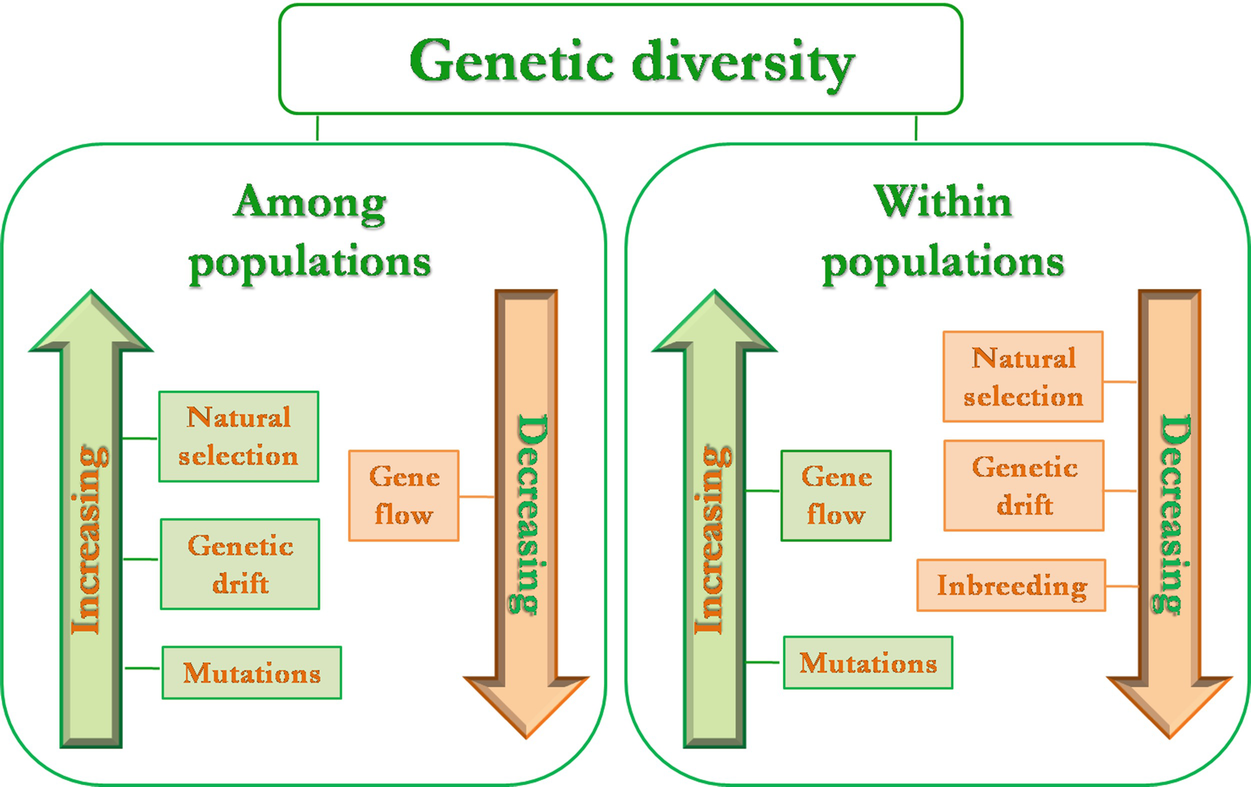
Mutation is the raw material generator. It's slow, random, and happens at roughly one new variant per replication cycle per genome. For large organisms with long generation times, mutation alone is basically irrelevant on any timescale that matters for conservation or agriculture. You won't see meaningful change from mutation without something else pushing it along. Recombination during sexual reproduction is where things get interesting. Every time meiosis happens, chromosomes swap segments. The shuffling itself doesn't create new alleles, but it creates new combinations of existing alleles, and that combinatorial explosion is what actually makes populations more diverse in practical terms. Outcrossing between related but not identical individuals will show a dramatic diversity spike in a single generation because the genotype space explodes even if the allele pool hasn't changed. Gene flow is the most potent lever you have. Migration and mating between previously isolated populations introduces entirely new alleles into a pool. This is why habitat fragmentation is such a destructive force, not just because it reduces population size but because it stops gene flow and lets drift quietly erode diversity over time. I've seen corridors designed and built for this purpose, and the results can be striking within two to three generations if the populations are still viable enough to actually move and breed.
What People Miss About Measuring Diversity
Heterozygosity is the go-to metric, but it saturates quickly. Once a population loses rare alleles through drift, heterozygosity doesn't reflect that loss accurately for a long time. Allelic richness, which counts the number of distinct alleles per locus, drops much faster and is a more honest signal of what's actually happening. If you're only measuring one or the other, you're flying partially blind. I used to work with microsatellite panels that were decent for individual identification but terrible for detecting recent bottlenecks because the loci were too polymorphic to show the signal. Switching to SNP arrays changed everything, but even then you have to think carefully about ascertainment bias. Arrays designed for domesticated populations often underperform when you're working with wild or semi-wild groups, and I've wasted money on datasets where half the markers were monomorphic in my study population.
Get the Full Details
When Diversity Isn't Actually Beneficial
This is the part nobody likes to talk about. Increased genetic diversity is not an automatic good in every context. Hybrid vigour or heterosis is real and well-documented, but it's not universal. In some cases, outcrossing between differentiated populations has led to outbreeding depression, where locally adapted gene combinations get broken apart and fitness actually drops. I was part of a project where we introduced fish from a nearby watershed into a threatened population and saw improved genetic metrics but reduced survival rates in the wild by roughly thirty percent over two years. The introduced alleles were maladapted to the specific stream conditions those fish were in. So the practical takeaway is that you need to think about adaptive variation, not just neutral markers. Genome-wide scans for selection signatures, landscape genetics approaches, and sometimes even controlled cross-breeding experiments before you commit to a management decision. It takes more work, obviously, but the cost of getting it wrong is measurable in lost individuals and wasted resources.
Practical Steps If You're Working With A Managed Population
Start by genotyping what you have before you do anything. You'd be surprised how many operations skip this and just manage on pedigree records, which are often incomplete or inaccurate by the second or third generation. Once you have baseline data, run a bottleneck analysis and calculate both heterozygosity and allelic richness across your loci. Then identify whether your main constraint is drift or isolation. If drift is the issue, you're managing population size and generation interval. If isolation is the issue, you're looking at gene flow interventions, whether that means physical corridors, translocations, or assisted reproductive techniques if the populations are too small to support natural movement. I've used frozen semen from stored samples to restore diversity in cases where live transport was logistically impossible or ecologically risky. It's not a perfect solution because you're limited to whatever genetic material happened to be preserved, but it beats watching a population erode. Monitor after every intervention. One round of gene flow doesn't fix a problem permanently, and without follow-up genotyping you won't know whether your moves are actually working or just looking good on paper. I usually set checkpoints at generation three and generation five for species with longer lifespans, and at each generational interval for faster-breeding organisms.