Diffusion and Passive Transport: What Actually Happens at the Membrane
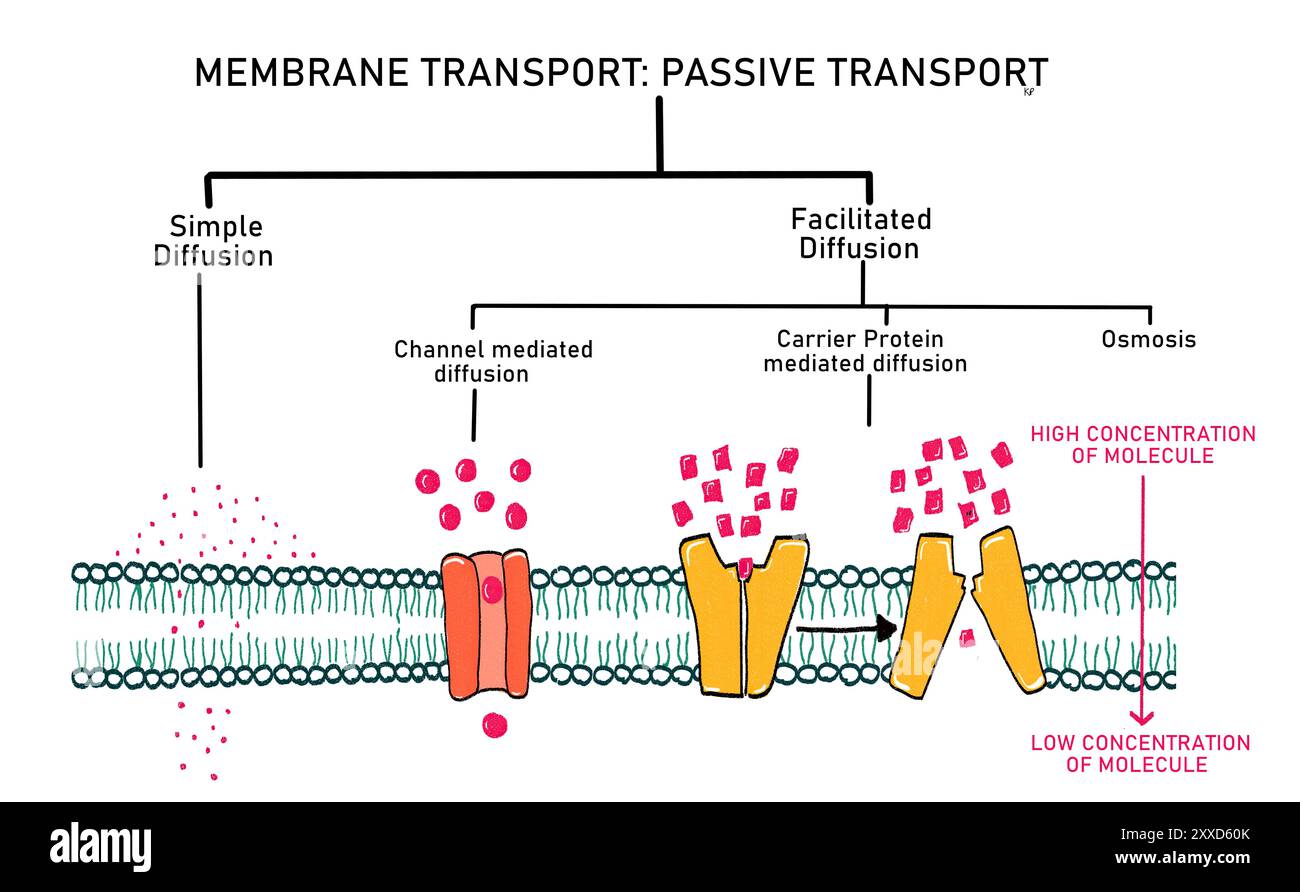
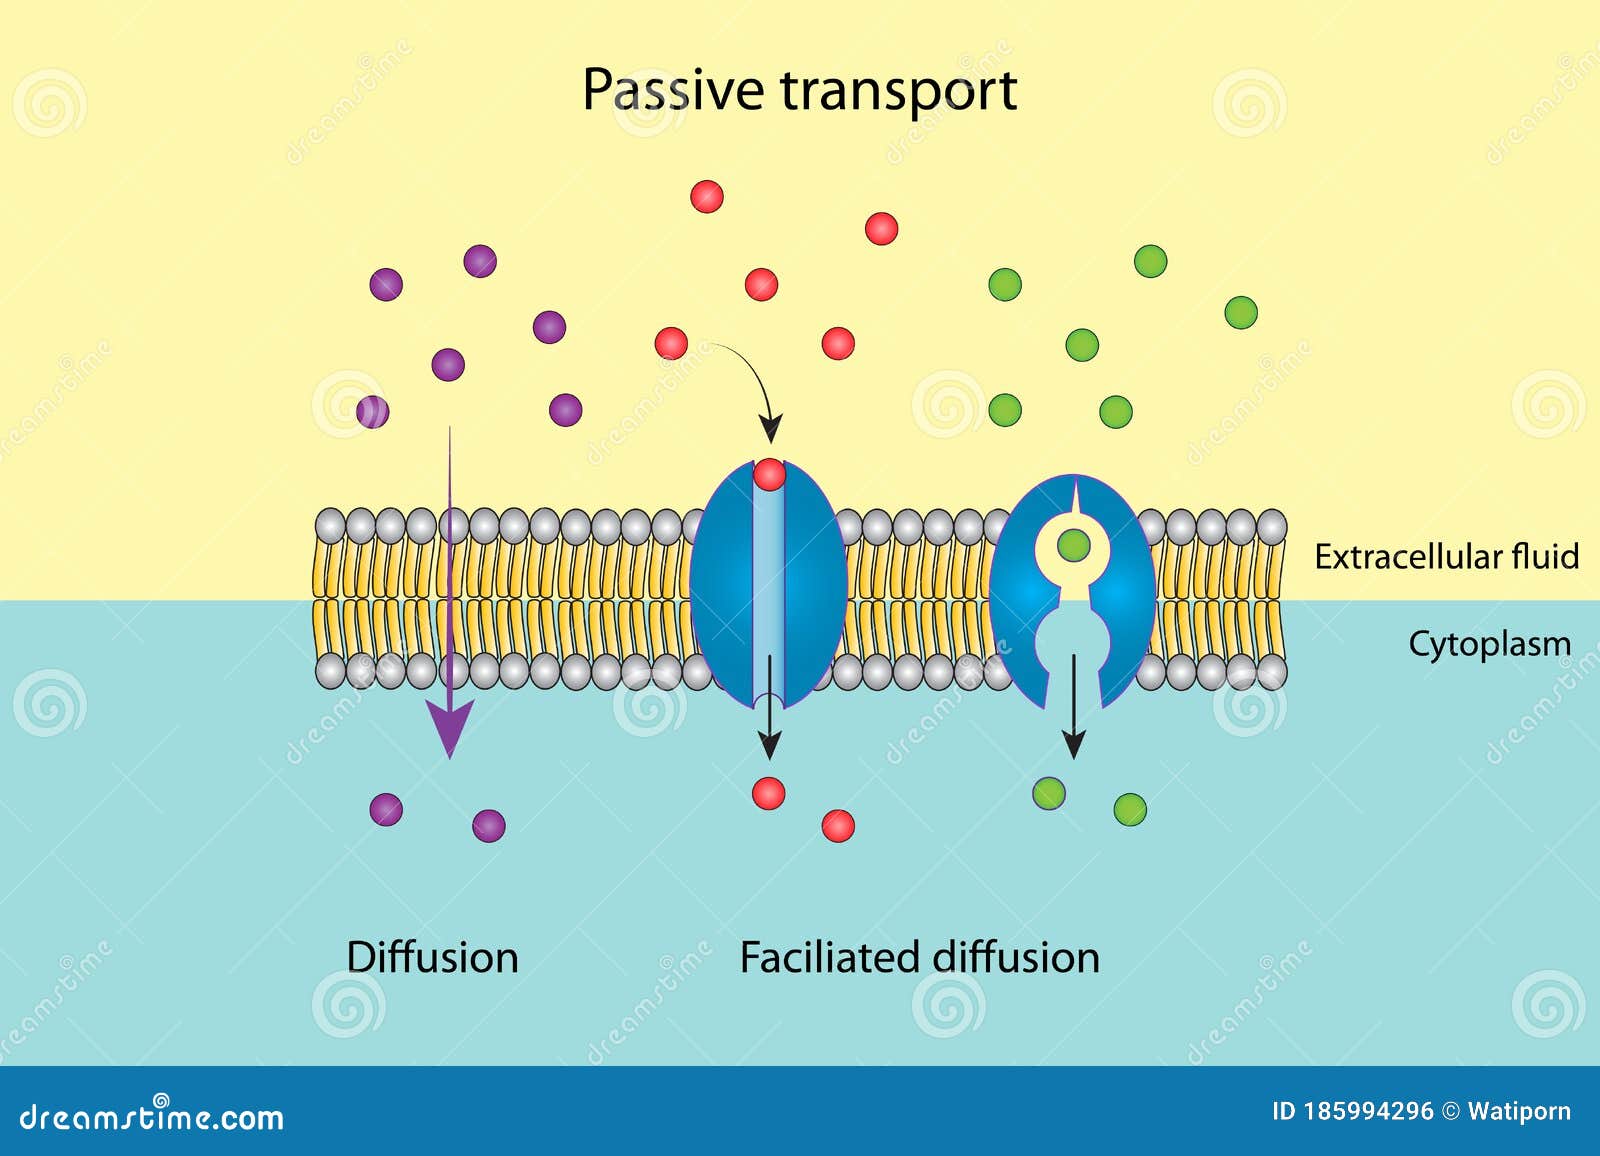
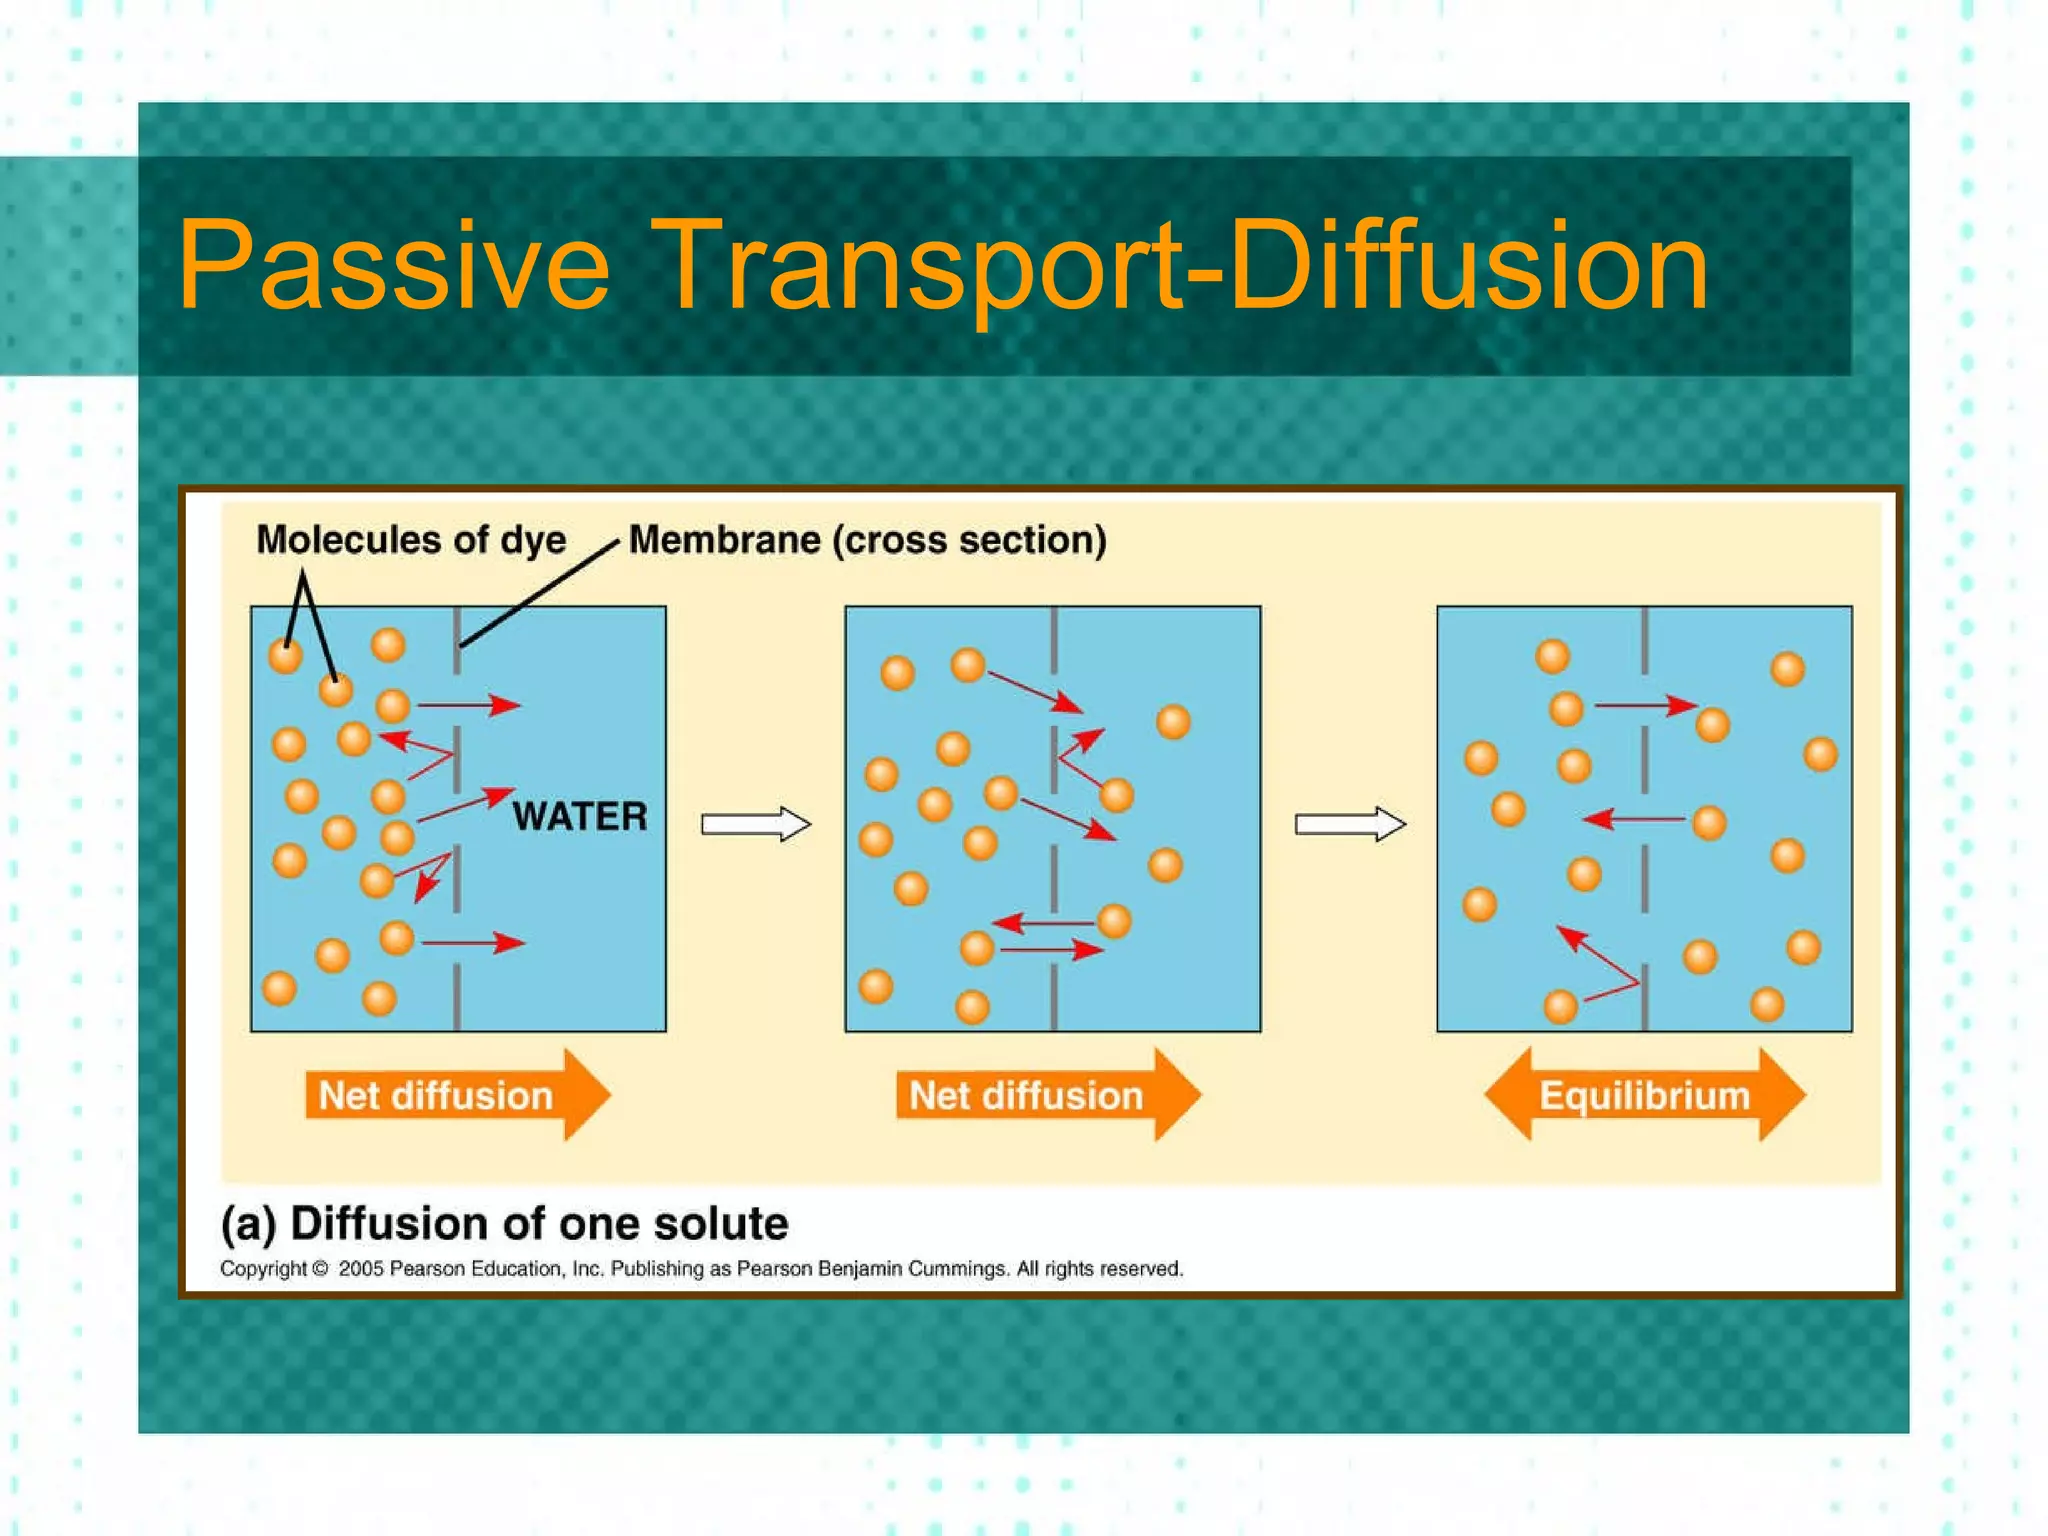
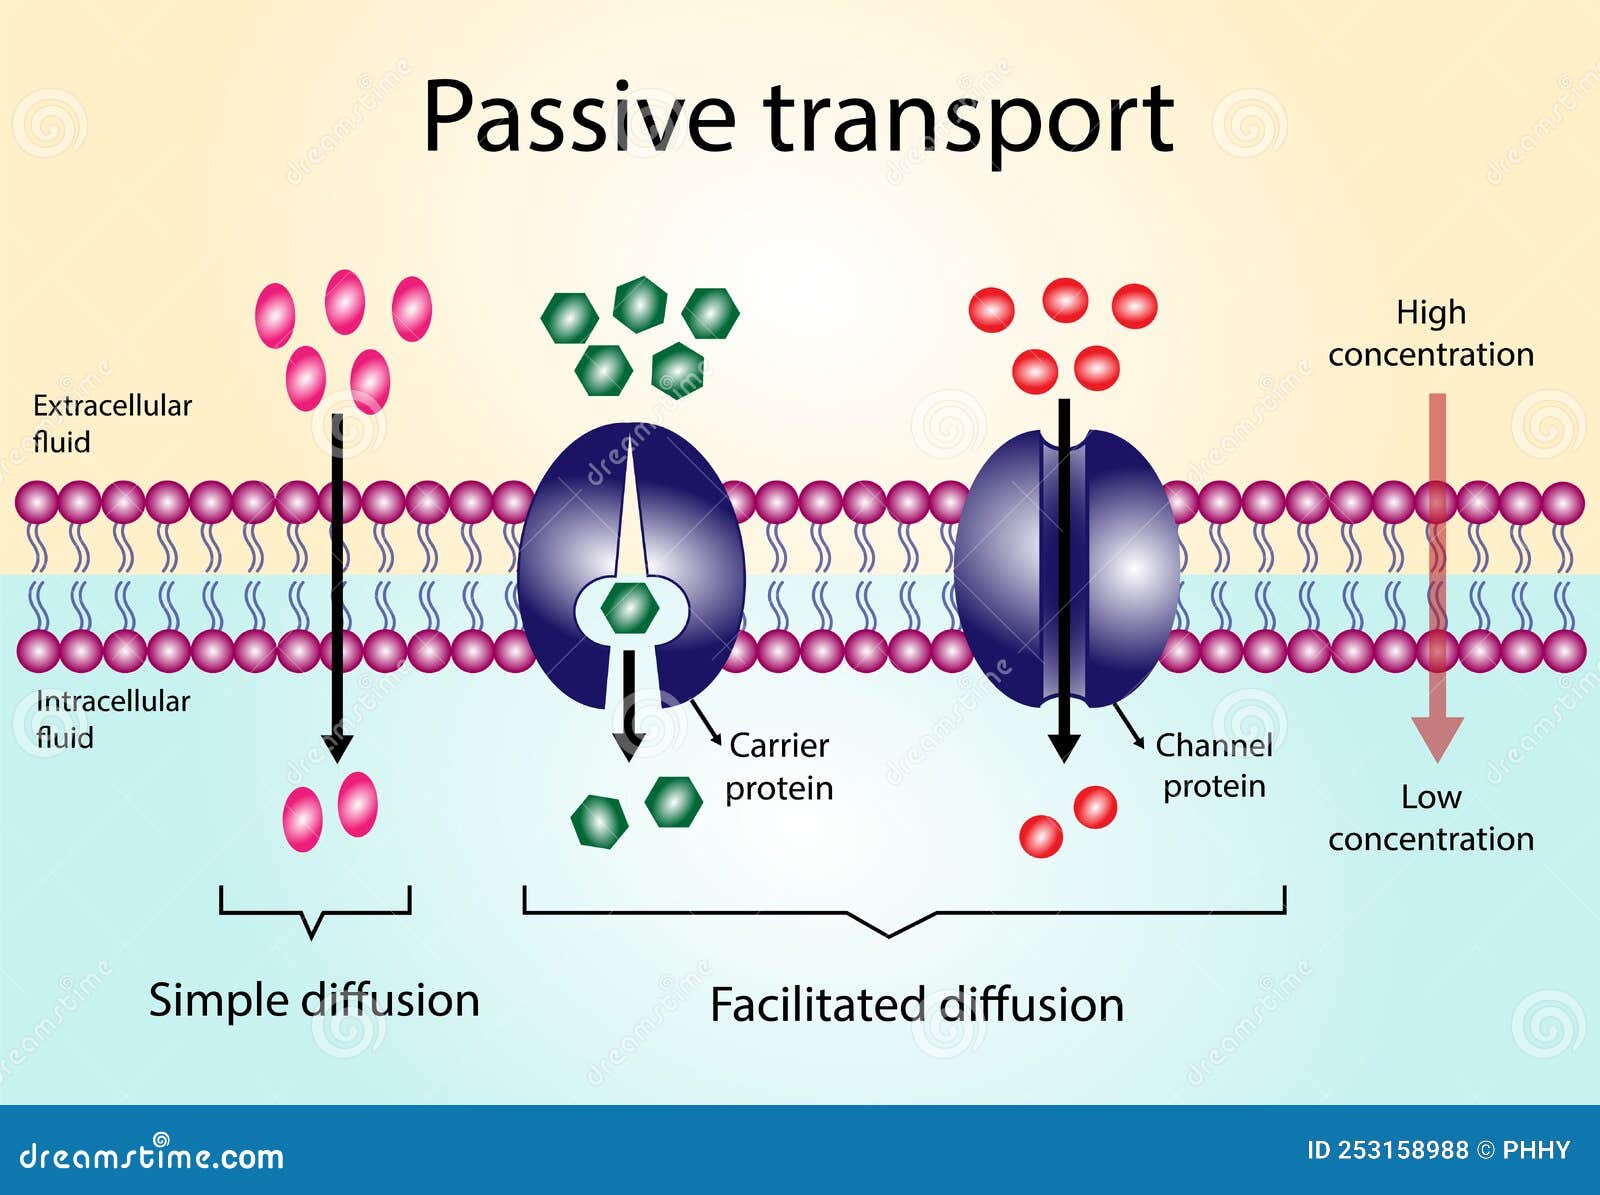
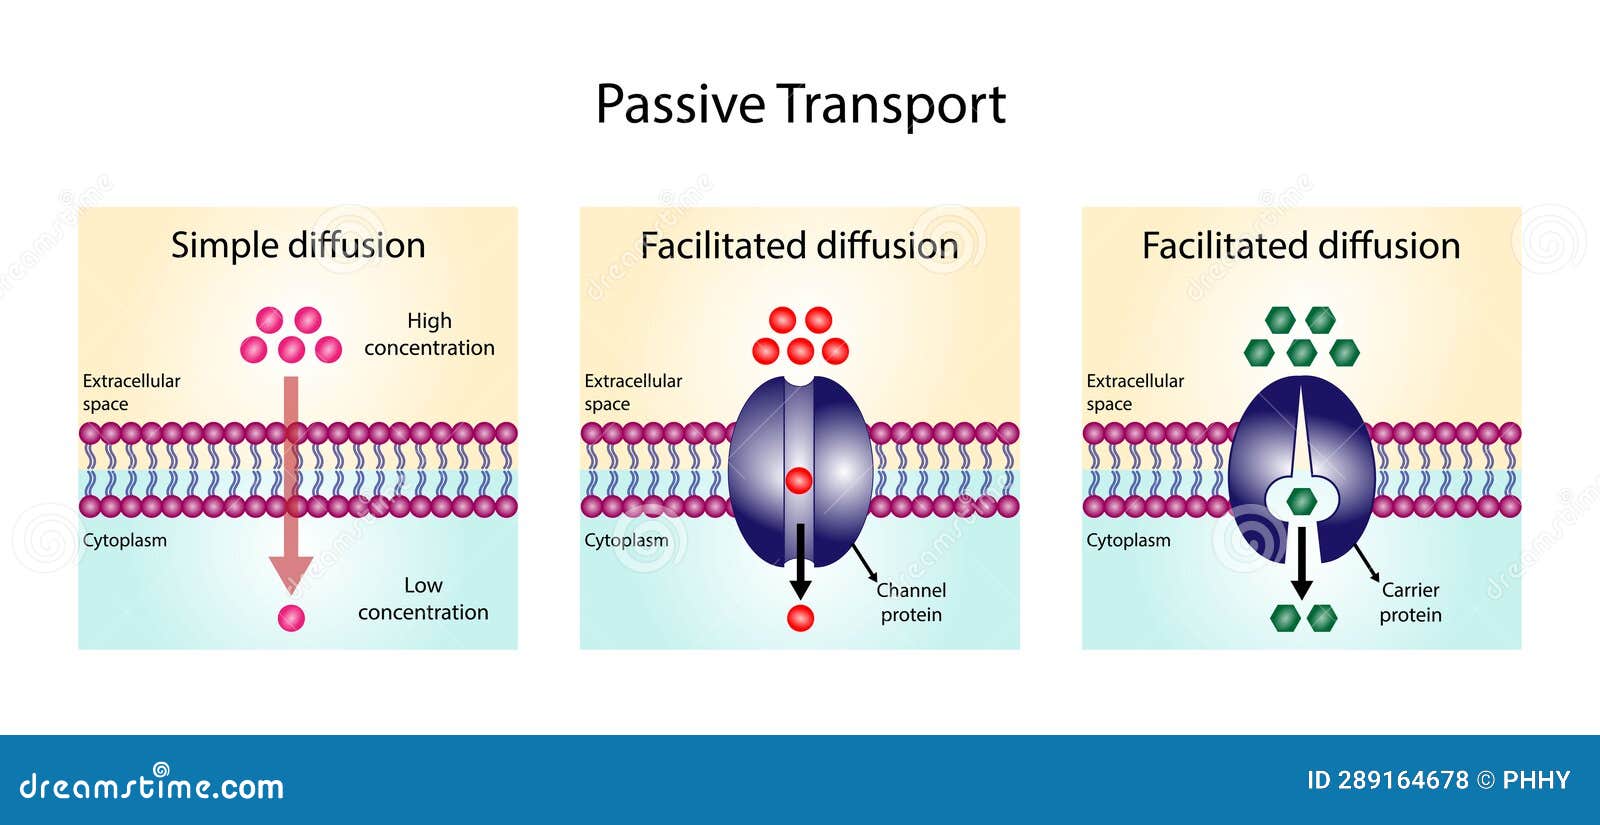
A lot of people get confused about whether diffusion counts as passive transport, usually because the terms overlap in different classes and textbooks aren't always consistent about it. Here is the straightforward breakdown of how it works, what the exceptions are, and where things tend to go wrong in practice. Diffusion is the net movement of particles from an area of higher concentration to an area of lower concentration. It happens because molecules are constantly in random thermal motion. When there is a concentration gradient, more molecules happen to move away from the concentrated side than toward it, simply by probability. That net movement is diffusion. Passive transport is any movement across a membrane that does not require cellular energy, meaning no ATP hydrolysis is involved. So yes, diffusion is passive transport, specifically the form that does not require a membrane protein at all. Facilitated diffusion is also passive transport because it still goes with the concentration gradient and uses no energy, but it requires a channel or carrier protein to get across the hydrophobic core of the lipid bilayer.
Is Diffusion Passive Transport
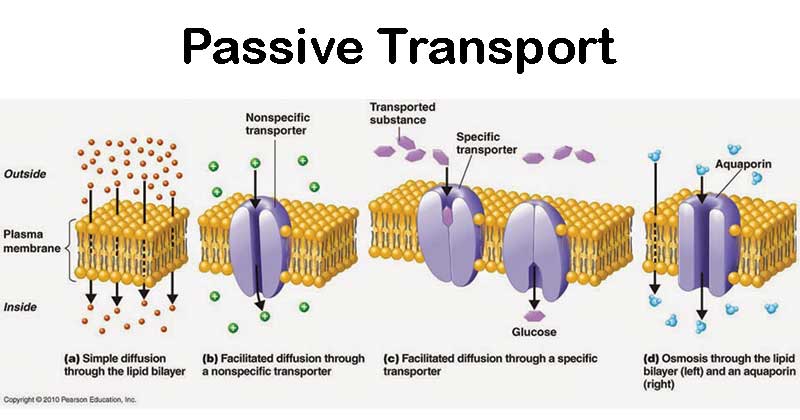
Short answer: yes. But the way people usually mess this up is by treating all diffusion as the same thing. It is not. Simple diffusion, osmosis, and facilitated diffusion are all passive, but they have very different kinetics and constraints, and you need to know which one you are dealing with before you model or predict anything. Simple diffusion applies to small, nonpolar molecules like oxygen, carbon dioxide, and nitrogen. These slip directly through the lipid bilayer because they are compatible with the hydrophobic interior. The rate depends on the concentration gradient, the surface area of the membrane, the thickness of the membrane, and the permeability coefficient of the molecule, which itself is determined by size and lipid solubility. Fick's first law describes this mathematically, but in practice what matters is that the driving force is purely the gradient. Once the gradient flattens out, net movement stops. I have seen students write lab reports claiming equilibrium means molecules stop moving entirely, which is wrong. At equilibrium, individual molecules are still bouncing around randomly in both directions, but the net flux is zero because the rates are equal. That distinction matters if you are doing anything with isotopic tracers or measuring actual particle trajectories. Osmosis is just the diffusion of water across a semipermeable membrane. The same principles apply, except water is polar and moves slowly through the lipid bilayer itself, so most cells rely on aquaporins to make it fast enough. Even with aquaporins, osmotic flow is still passive. No ATP, no coupling to another gradient. Just water following its own chemical potential gradient, which in biological systems is usually expressed as an effective osmolarity difference across the membrane.
Facilitated diffusion uses transmembrane proteins, either channels or carriers, to move substances down their gradient. Glucose entering red blood cells through GLUT1 is the classic example. The key thing most people miss here is that facilitated diffusion is saturable. Unlike simple diffusion, where rate increases linearly with concentration indefinitely, facilitated diffusion follows Michaelis-Menten-like kinetics because there are a finite number of transporters. At low substrate concentrations, the rate looks almost linear, but as concentration rises, the transporters get occupied and the rate plateaus. I ran into this explicitly when I was modeling glucose uptake in a cell culture system and the uptake rate didn't scale up the way the simple diffusion equation predicted at higher concentrations. The fix was switching to a carrier-mediated kinetic model with a Vmax parameter instead of relying on Fick's law. Once I did that, the fit was solid. Ions are a separate category that people often lump in incorrectly. Simple diffusion of ions through the lipid bilayer is essentially zero because the charged species cannot shed their hydration shell to enter the hydrophobic core. Ions move through channels, and whether that counts as simple diffusion or something more nuanced depends on what you are tracking. Voltage-gated and ligand-gated channels are still passive in the sense that the ion moves down its electrochemical gradient without direct ATP input. But the gradient itself is maintained by active pumps like the Na+/K+-ATPase, so ion movement through channels is indirectly dependent on active transport keeping the gradients alive. That causal chain is easy to gloss over in an intro class and hard to catch when your experimental data does not match the prediction. The biggest practical pitfall I see is assuming that because a process is passive, it cannot be regulated. Facilitated diffusion is absolutely regulated. Channel gating, transporter expression levels, membrane composition, and even the lipid environment around the transporter all affect the rate. A membrane with more cholesterol will be less permeable to small nonpolar molecules than one with less, which changes the diffusion coefficient. Temperature matters too, since diffusion is fundamentally a kinetic phenomenon. In my own work, I once forgot to control for temperature when comparing diffusion rates across two membrane preparations and spent about three days trying to figure out why the data were inconsistent before realizing the incubator had drifted by four degrees Celsius.
Get the Full Details
Another thing that is not obvious is that diffusion is only useful over short distances. The time it takes for a molecule to diffuse scales with the square of the distance. A molecule diffusing across a single cell membrane, say 10 nanometers, takes microseconds. Across a millimeter, it takes minutes. Across a centimeter, it takes hours or days. This is why multicellular organisms need circulatory systems and why neurons have active transport mechanisms along microtubules for moving cargo over long axonal distances. Diffusion alone would not keep up. If you are trying to determine experimentally whether a transport process is passive diffusion or something else, the standard approach is to measure uptake or flux across a range of external concentrations and see if the kinetics are linear or saturable. Linear kinetics suggest simple diffusion. Saturable kinetics suggest carrier-mediated transport. You can also test for temperature sensitivity, though both simple and facilitated diffusion show some temperature dependence because viscosity and molecular motion change with temperature. The more definitive tests involve using specific inhibitors for known transporters or knocking down channel expression to see if flux drops, which rules out simple diffusion through the lipid bilayer. There are also cases where the distinction gets blurry. Some molecules exhibit both simple and facilitated diffusion simultaneously. A compound might pass through the lipid bilayer slowly by simple diffusion while also being transported by a specific carrier. The total flux is the sum of both pathways, and untangling them requires careful experimental design. I encountered this with a lipophilic drug compound where the apparent permeability in a cell monolayer assay was higher than what the lipid solubility alone would predict, and the excess flux was eliminated when we blocked the organic anion transporting polypeptide that was also handling the compound.
The bottom line is that diffusion is passive transport, but calling it passive transport tells you almost nothing about the mechanism. You need to know whether it is simple diffusion, osmosis, or facilitated diffusion, because each has different constraints, different kinetics, and different regulatory points. And in practice, biological membranes are complicated enough that the textbook ideal cases rarely show up in isolation.