Understanding Mitochondria Across Cell Types
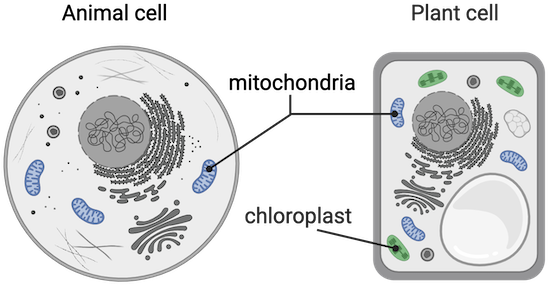
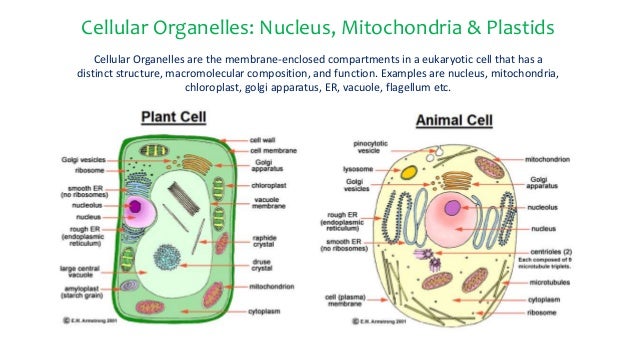
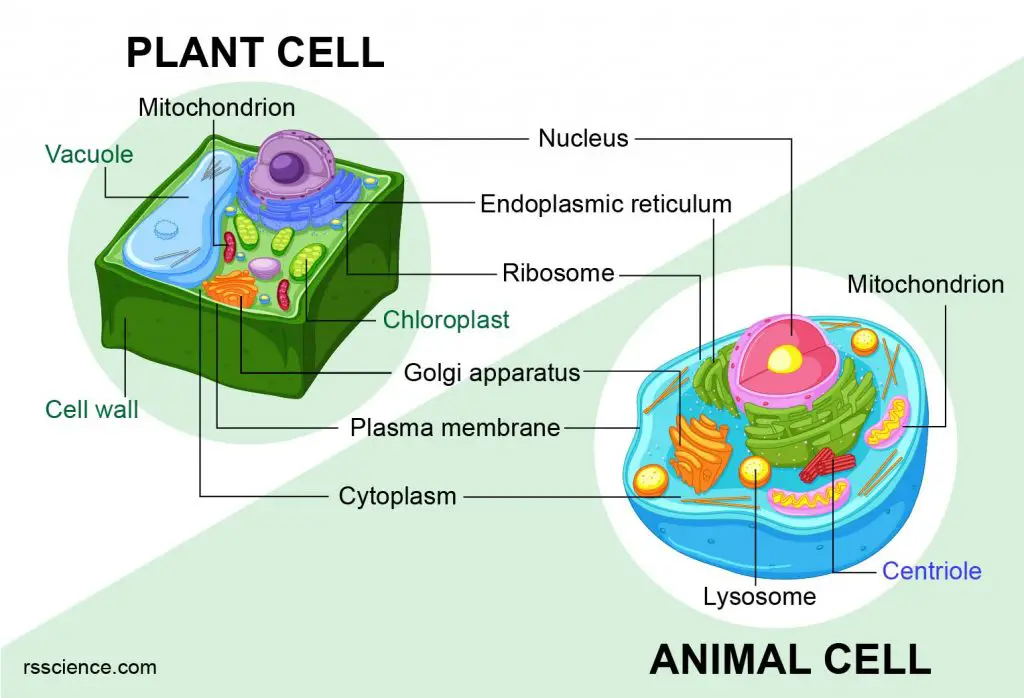
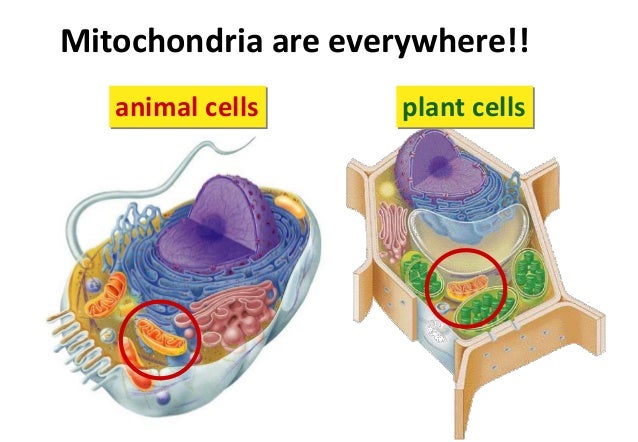
Most introductory biology resources treat mitochondria as a single generic thing, which works fine for high school exams but breaks down fast once you start working with actual tissue samples. The reality is that mitochondria behave quite differently depending on their cellular context, and the differences matter if you care about accurate experimental results or just understanding how these organelles actually function. The short answer is yes, both plant and animal cells contain mitochondria. This is not controversial. What people often miss is that having mitochondria doesn't mean the same things are happening inside them. Plant mitochondria have fundamentally different metabolic roles compared to animal mitochondria, and they operate under different constraints entirely. Here's something most people don't realize: plant mitochondria are generally larger than animal mitochondria, but plant cells contain significantly fewer of them. A typical mammalian cell might have anywhere from a thousand to several thousand mitochondria depending on energy demand, while a plant cell usually carries only a few hundred. This isn't because plants don't need energy — it's because plant cells also run photosynthesis, which generates ATP directly in the chloroplasts during daylight hours. The mitochondria in plant cells end up sharing the load rather than being the primary power source.
Another thing that comes up frequently is the alternative oxidase pathway. In animal cells, the electron transport chain pushes protons across the inner membrane to drive ATP synthase, and that's basically the only show in town. Plant mitochondria have an extra escape hatch called alternative oxidase that lets electrons bypass complexes III and IV entirely. This means protons don't get pumped, no ATP is made, but the energy gets released as heat instead. This matters for certain plants that need to thermogenize to volatilize scent compounds or melt through frost. It's an entirely different use case from what animal mitochondria are doing. When I was sequencing mitochondrial genomes for a comparative study a few years back, I hit a wall with plant samples that completely derailed my timeline. Plant mitochondrial genomes are massive compared to animal ones — I'm talking 200 kilobases to over 11,000 kilobases in some species, versus the tidy 16,569 base pairs we see in human mtDNA. But here's the real problem: those genomes are highly dynamic. They undergo frequent recombination between small repeat sequences, which generates multiple structural isoforms simultaneously within a single cell. When you extract plant mitochondrial DNA and throw it at a standard short-read assembler, you get a mess of conflicting contigs that look like the genome is falling apart. It's not falling apart — it's just doing what plant mitochondrial genomes naturally do. The workaround I ended up using was switching to long-read sequencing with the Oxford Nanopore platform. Yes, the error rate is higher per base, but with the read lengths available, you can span those repeat regions and resolve the actual genome structure. For plant mitochondrial genomes specifically, I found that targeting roughly 50x coverage on a MinION flow cell gave me assemblies I could trust. Short-read Illumina data alone just couldn't handle the repetitive landscape. If you're working with animal mitochondrial genomes, this problem essentially doesn't exist — they're small, conserved, and assemble cleanly with pretty much any technology.
Isolation procedures differ significantly between the two as well. Plant cell walls make mechanical homogenization a nuisance. You need a pre-softening step, usually involving cellulase and pectinase digestion, to break down the wall without shearing the organelles apart. I spent weeks optimizing buffer conditions for liver tissue isolation before someone pointed out that leaf tissue needs an entirely different approach. The sucrose gradient centrifugation ratios shift because plant mitochondria have different buoyant densities, and chloroplast contamination is a persistent problem unless you layer your gradients carefully. There's also a functional nuance worth noting. Animal mitochondria are heavily optimized for oxidative phosphorylation efficiency. Plant mitochondria sacrifice some of that efficiency for regulatory flexibility. This is why inhibitors like cyanide, which block cytochrome c oxidase in animals and are essentially fatal, only partially affect plant respiration. The alternative oxidase pathway takes over and keeps things running. If you're doing pharmacological experiments with mitochondrial inhibitors, applying animal-derived concentration ranges to plant tissue will give you misleading results. The dose-response curves are completely different. One more thing that trips people up: the inheritance patterns. Animal mitochondrial DNA is almost universally maternally inherited. Plant mitochondrial DNA inheritance is far more variable — it can be maternal, paternal, or biparental depending on the species. In some conifers, for example, mitochondria are paternally inherited through the pollen, which is the opposite of what you'd expect if you only studied animal models. This has real consequences for population genetics work and phylogenetic studies that assume a single mode of inheritance.
Get the Full Details
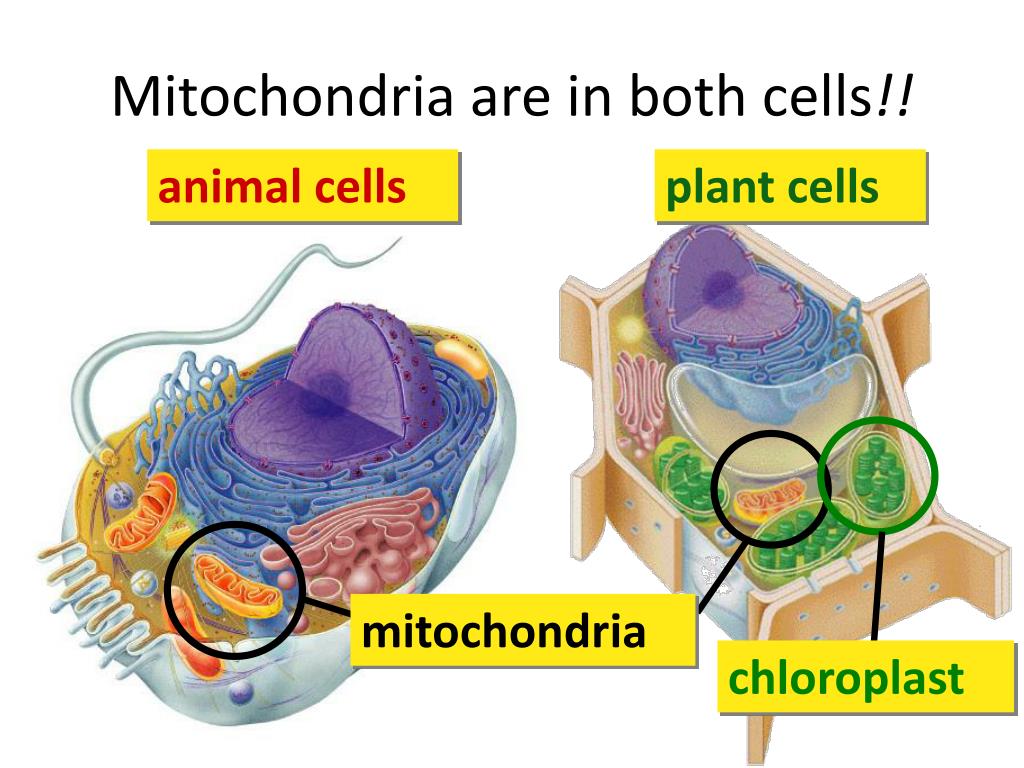
If you're new to working with these organelles, the biggest mistake I see is treating them as interchangeable. They share the same basic architecture — double membrane, cristae, their own circular genome, ribosomes that resemble bacterial ones — but beyond that structural similarity, the functional divergence is significant enough that protocols and assumptions don't transfer cleanly between plant and animal systems. Spend time understanding the differences before running a one-size-fits-all protocol and wondering why your yields are poor or your data looks weird.