Understanding Reproductive Strategies in Ecology
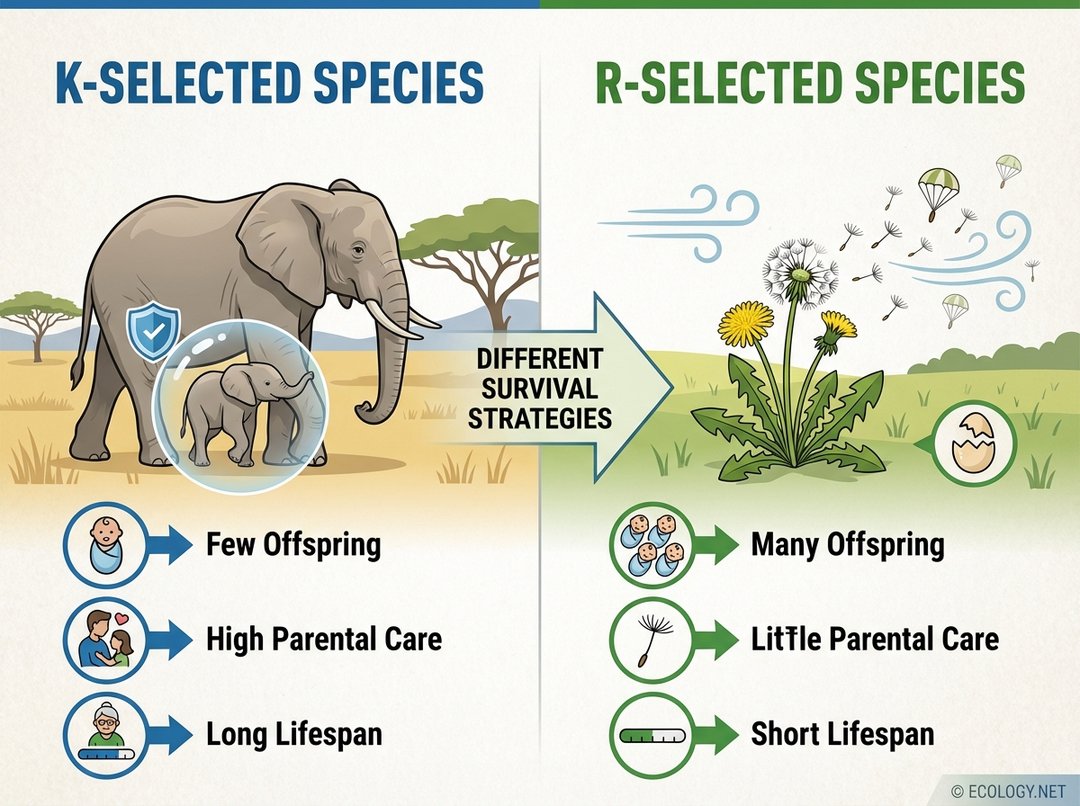
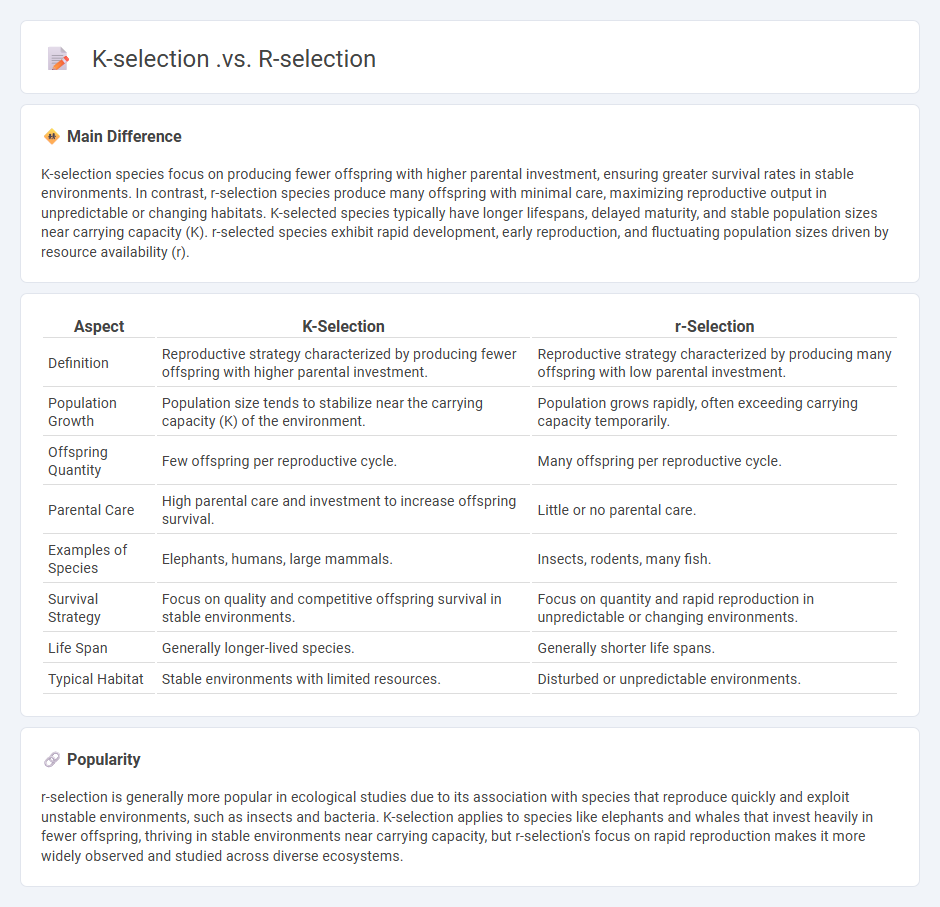
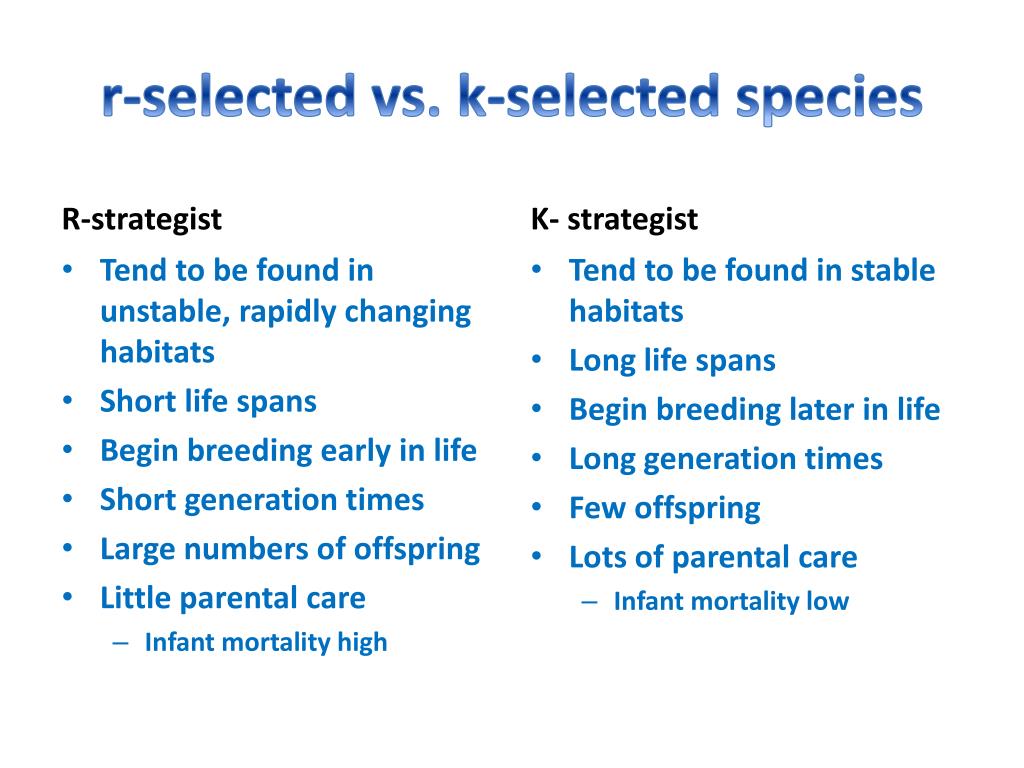
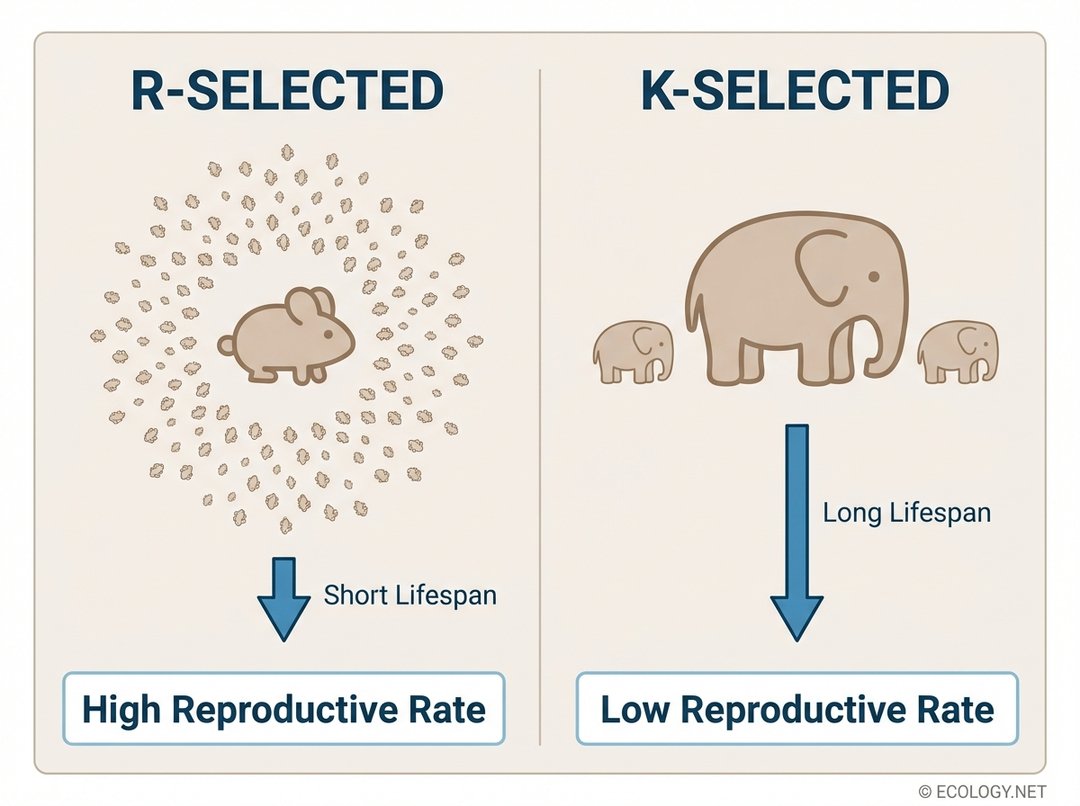
Most people encounter the K Selected Vs R Selected framework in an introductory biology course and think they've got it figured out. The textbook version is simple enough: r-strategists produce lots of offspring with little investment, while K-strategists produce few and invest heavily. That's accurate on paper. It's also not particularly useful when you're actually working with real ecosystems. The original framework comes from MacArthur and Wilson's 1967 work on island biogeography, but ecologists have been refining and critiquing it for decades. Before I get into the mechanics, here's something that trips people up constantly: the r/K dichotomy is a spectrum, not a binary. Almost no organism sits at either extreme. Humans, elephants, and whales are K-dominant, sure. But even kelp, which lays millions of eggs, isn't a pure r-strategist because the environment does much of the parent-investment work through nutrient provisioning in the egg itself.
How to Classify a Species Using the K Selected Vs R Selected Framework
The classification process starts with life history parameters, not behavioral observations. You need data on age at first reproduction, clutch or litter size, frequency of reproductive events per year, and estimated adult mortality rates. When I was grading undergraduate research projects on local freshwater fish populations, one student tried to classify a species based entirely on whether it "looked fragile." That's not how this works. Here's the practical workflow. First, compile age-specific survival and fecundity schedules from published literature or your own field data. Second, calculate the net reproductive rate (R0) and generation time (T). Third, compare your species against known benchmarks in the same taxonomic group. R-selected species typically show R0 values well above 100 with generation times under two years. K-selected species often have R0 near 1 to 3 with generation times measured in decades. I ran into a specific edge case last year while studying amphibian populations in the Piedmont region. We had a pond-breeding salamander species that produced only 40 to 60 eggs per clutch — clearly on the lower end for amphibians — but the adults had near-zero annual survival due to road mortality. That should make it K-selected by the numbers, but the population dynamics behaved like an r-strategist because the high adult mortality selected for rapid reproduction. The workaround was to stop using the r/K labels and switch to fast-slow continuum analysis using Pace-of-Life Syndrome metrics. That gave us actual predictive power instead of a misleading classification.
The Counter-Intuitive Parts Nobody Teaches
One thing that consistently surprises students is that r-selection doesn't guarantee population growth. In density-dependent environments, high reproductive output can be completely offset by competition among the offspring. I've seen graduate students treat r-selected species as inherently "successful" or "superior," which reflects a fundamental misunderstanding of the framework. These strategies are context-dependent adaptations, not hierarchies. Another overlooked nuance involves phenotypic plasticity. Many organisms can shift their position along the r/K continuum depending on environmental conditions. Daphnia, for example, will alter their clutch sizes and development rates in response to predator presence and food availability. This plasticity means a single species can exhibit both r-like and K-like strategies within its lifetime. The framework wasn't designed to handle this, and forcing these organisms into rigid categories creates analytical errors.
Get the Full Details
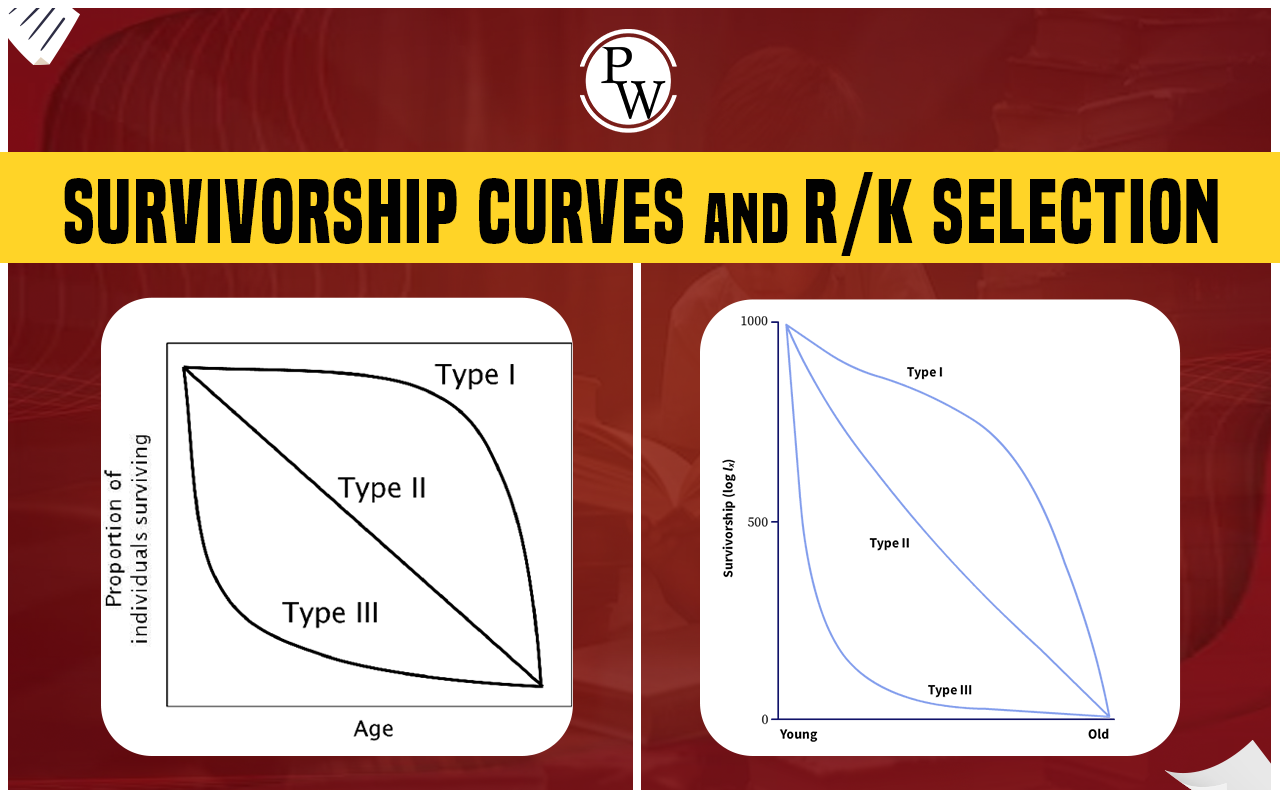
When the Framework Falls Apart
There are entire clades where the r/K selection model provides little explanatory value. Marine invertebrates with complex life cycles, certain parasitic plants, and many tropical tree species don't fit cleanly into either category. In these cases, alternative frameworks like Stearns' life history trade-off models or Reznick's demographic approaches give you more tractable predictions. The biggest limitation is that r and K were originally mathematical parameters from the logistic growth equation, not evolutionary strategies. Conflating the equation parameters with selective pressures leads to circular reasoning. When you see papers claiming "r-selection favors genotype X because r is high," that's often the model being used to explain itself rather than generating independent predictions. If you need a more robust classification system for conservation or management purposes, consider using the Collaborative Conservation Framework's life history trait database or the compendium of vertebrate life history traits compiled by Purvis and Hector. These resources pull from peer-reviewed sources and let you cross-reference multiple axes of variation simultaneously rather than collapsing everything into a single r/K axis.
Practical Application for Field Researchers
When you're actually in the field trying to assess whether a population is functioning under r or K dominated conditions, focus on three measurable indicators: juvenile survival rate, age at maturity relative to maximum lifespan, and population variability over time. R-dominated populations show high variance in abundance year to year. K-dominated populations hover closer to carrying capacity with smaller fluctuations. I found that collecting mark-recapture data over at least three complete reproductive cycles gives you enough signal to distinguish between the strategies with reasonable confidence. One or two seasons of observation will almost always leave you ambiguous, especially in temperate zones where interannual climate variation can swamp the underlying life history signal. The original MacArthur-Wilson formulation assumed closed populations on islands, which means you'll need to adjust your expectations when applying this to mainland systems with migration, seasonal variation, and complex community interactions. The framework still works as a starting point, but treating it as anything more than a heuristic will get you in trouble.