Working With Dihybrid Crosses When Things Don't Go According to the Books
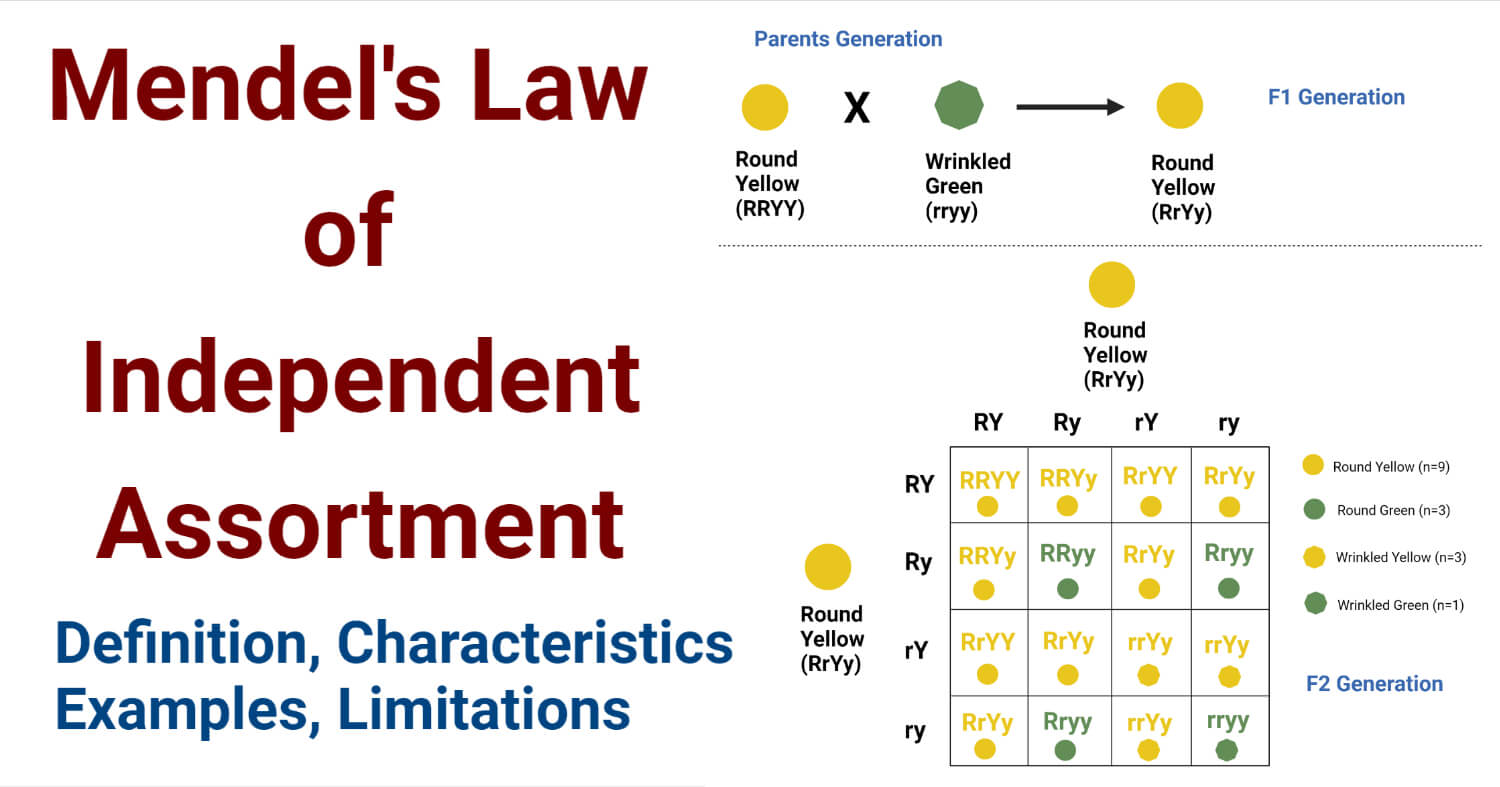
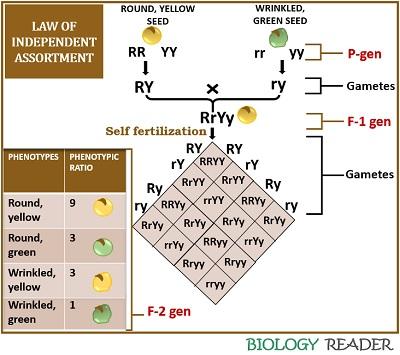
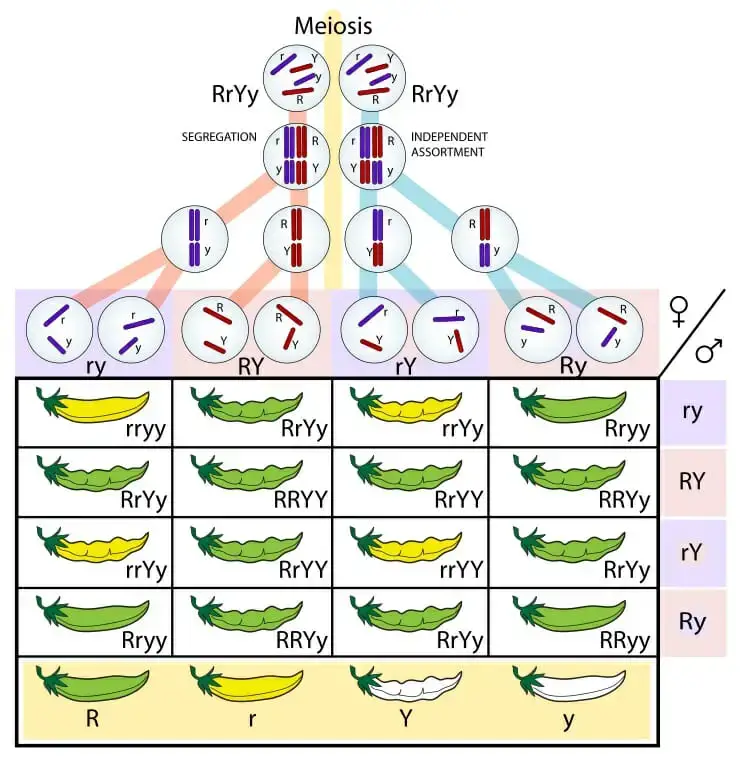
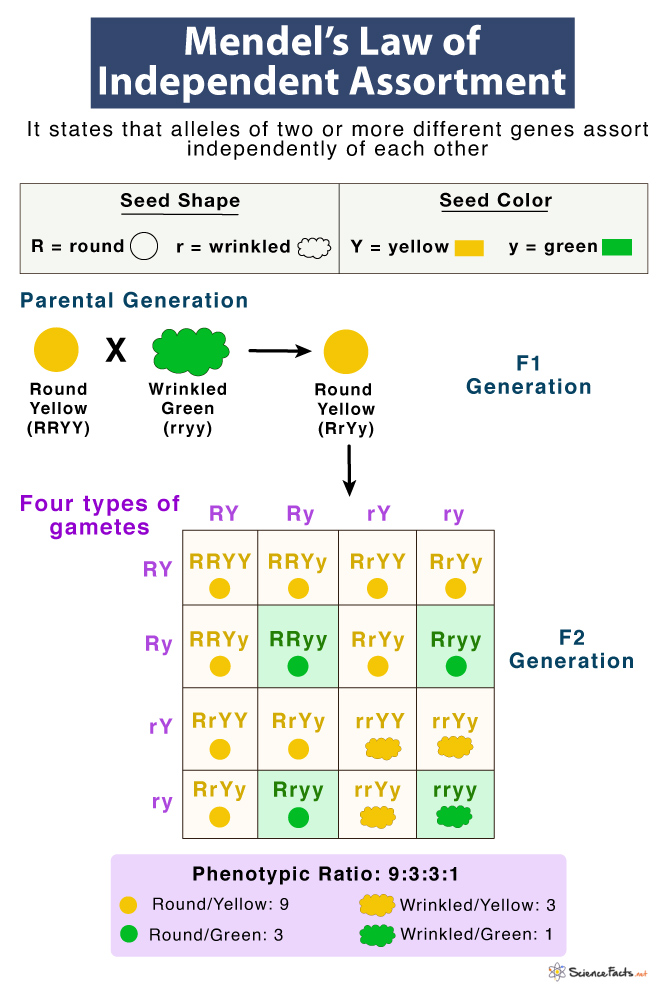
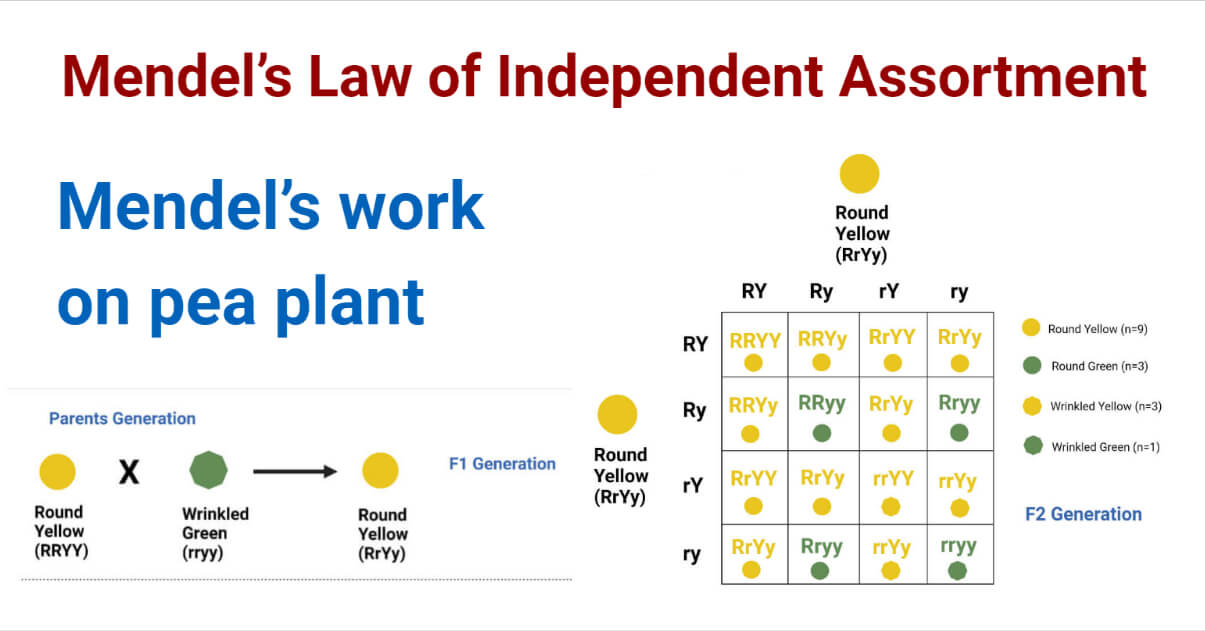
I spent years dealing with genetics problems in undergrad and then again when I was teaching intro bio labs, and the law that trips people up most isn't segregation at all. It's independent assortment. Specifically, Mendel S Law Of Independent Assortment sounds clean on paper but real chromosomes don't always behave that nicely. Independent assortment means alleles for different traits sort into gametes independently of one another. When you cross two organisms that differ in two traits, like seed shape and seed color in peas, you get that classic 9:3:3:1 ratio in the F2 generation. The dominant and recessive alleles for one trait have no say in how the alleles for the other trait end up in a gamete. That's the textbook version. The mechanism behind it is metaphase alignment during meiosis I. Homologous chromosome pairs line up at the equatorial plate randomly. The maternal and paternal chromosomes of each pair orient independently of every other pair. That's physical. That's why the math works.
But here's where the rubber meets the road. I once had a grad student bring me data from a pea cross that looked nothing like 9:3:3:1. We'd set up the cross exactly by the book. Two heterozygous parents, RrYy times RrYy. She counted about 400 F2 seeds and the ratio was closer to 6:3:3:2 with a big skew toward the double recessive class. She was convinced she'd made a counting error. I had her pull out the parental lines and verify the genotypes first. Turns out the Y allele in her stock was linked to a recessive lethal variant on the same chromosome. The chromosomes weren't assorting independently because the two loci were only about 8 map units apart on chromosome 4. She was measuring linkage, not independent assortment. That happened to me three or four more times across a decade of teaching. The problem always traces back to one thing: assuming two genes are on different chromosomes or far enough apart on the same chromosome without checking recombination frequency first.
When the Model Breaks Down
Independent assortment only applies to genes on different chromosomes or genes that are sufficiently far apart on the same chromosome. If two loci sit within roughly 50 centimorgans of each other, they show linkage and the expected gamete ratios shift. You'll see more parental type gametes and fewer recombinant types. The further apart they are, the closer you get back to independent ratios, but even at 40 cM you're still noticeably off. A common mistake students make is using a Punnett square for a dihybrid cross and writing out all 16 boxes without calculating whether the genes are actually unlinked. The square itself is fine for showing combinations, but if the underlying assumption of independent assortment is wrong, the whole thing predicts garbage. I've seen people use these squares for human pedigree analysis on genes known to be linked. It doesn't work. Period. Another thing that gets overlooked is sex linkage. If one of your traits is on the X chromosome, males and females will show different phenotypic ratios in the F2 generation. Independent assortment still technically happens for the autosomal gene, but the overall ratio gets distorted because the sex chromosome doesn't segregate the same way in XY systems. If you're working with Drosophila or any organism with heterogametic males, flag that immediately before you start calculating ratios.
Get the Full Details
How to Verify Whether Genes Are Really Assorting Independently
Don't just assume. Run a test cross. Mate the dihybrid individual to a homozygous recessive partner and count the offspring classes. If you're getting roughly equal numbers across all four phenotypic categories, the genes are unlinked. If two categories dominate and the other two are significantly reduced, you've got linkage. A chi-square test against the 1:1:1:1 expectation for a test cross will tell you statistically whether deviation from independence is real or just sampling noise. For classroom work where you can't actually do crosses, look up the genes in a genome browser or a genetic map database. Checking whether two loci share a chromosome and what their reported recombination fraction is takes about two minutes and saves you from building an entire problem on a false premise. I always tell my students to do that check before they write a single Punnett square. It has cut down on wasted lab time significantly.
A Practical Approach That Actually Works
When you're solving a problem and you need to apply Mendel S Law Of Independent Assortment, follow this order instead of jumping straight into a 16-box grid. First, confirm the chromosomal location of each gene. Second, determine the genotype of each parent. Third, calculate gamete frequencies using recombination data if linkage exists, or use the simple half-half split per locus if genes are unlinked. Fourth, combine gamete frequencies using the multiplication rule. Fifth, convert to phenotypic ratios only after you have the genotype frequencies locked in. The multiplication rule is where most shortcuts fail. If you know one locus gives you a 3:1 phenotypic ratio and the other also gives 3:1, you multiply (3:1) times (3:1) to get 9:3:3:1. That only works when the loci are independent. If there's any linkage, you can't do that shortcut. You have to go through the gamete step explicitly. I keep a simple reference sheet for common model organisms with mapped locations for the standard lab genes. For peas it's not too bad since Mendel's seven traits are scattered across different chromosomes. For maize or Arabidopsis it gets messier quickly. But having that reference avoids at least half the errors I see in student work.
Where This Approach Falls Short
Independent assortment is a model, not a universal law. It fails whenever genes are linked, which is most of them in practice since genomes have finite chromosome numbers. It also fails with epistasis, where one gene masks or modifies the expression of another. Epistasis doesn't break the chromosomal mechanics, but it completely changes the phenotypic ratios you'd predict from independent assortment alone. A 9:3:3:1 genotypic framework can turn into 9:7 or 12:3:1 or any number of modified ratios depending on the interaction. There's also meiotic drive, where certain alleles bias their own transmission during gamete formation. That's rare in standard lab organisms but well documented in some natural populations. Independent assortment assumes fair meiosis. Meiotic drive breaks that assumption. If you're working with wild populations or non-model organisms, you should expect deviations more often than you would in a controlled lab cross. For most introductory purposes the model holds well enough. But if you need accurate predictions for breeding programs or genetic counseling, you move beyond Punnett squares into linkage maps, haplotype phasing, and probabilistic simulation. Those tools account for the fact that chromosomes, not abstract gene symbols, are what actually get shuffled.