Working With Model Organisms When the Literature Doesn't Match Your Bench
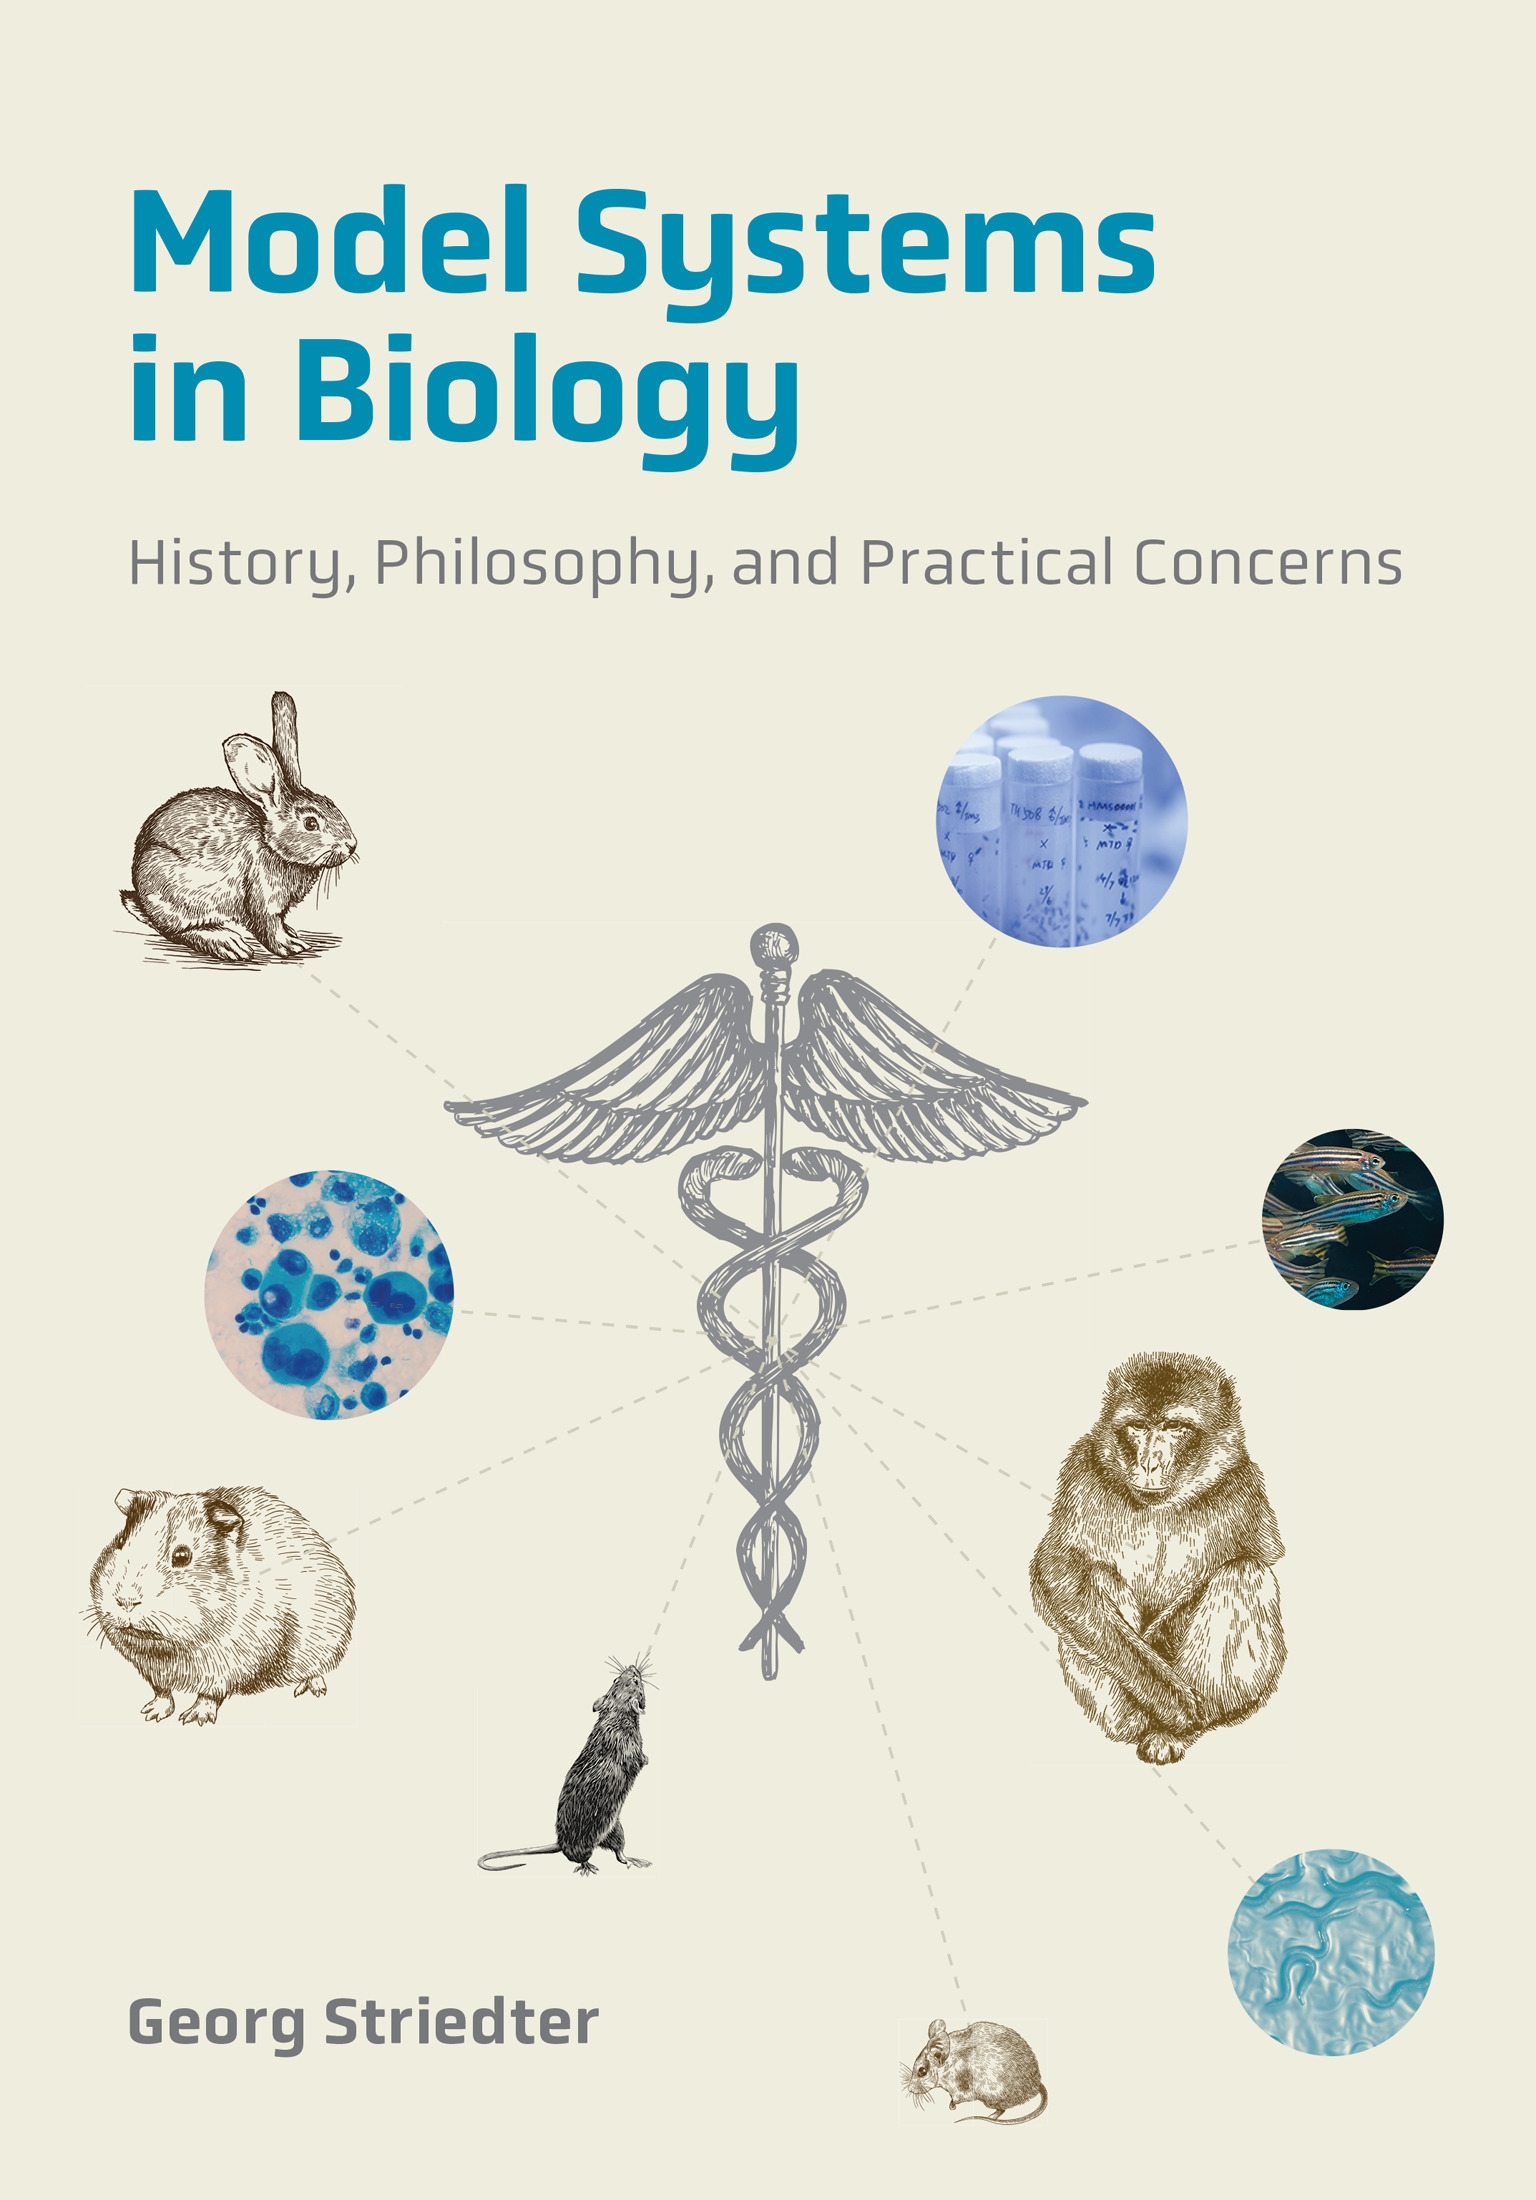
Most people treat a model system as if it comes with a user manual that actually applies to their particular experiment. That assumption breaks down fast. The organism itself is only as useful as the specific strain, growth conditions, and experimental window you have going. A model system in biology is an organism chosen because it has practical features that make certain kinds of research possible. It is not a perfect stand-in for humans or even for other organisms in your field. It is a tool with a narrow set of reliable properties.
Model System In Biology: The Short Definition Nobody Uses Honestly
The formal definition says a model organism is a non-taxonomically significant species heavily studied to understand particular biological processes. That misses the actual selection pressure. Researchers pick model organisms for repeatability, short generation time, available genetics, and institutional support. Everything else is secondary. Drosophila melanogaster stays dominant because the genetic toolkit is enormous. Arabidopsis thaliana stays around because it is cheap and easy. Caenorhabditis elegans is used because nearly every cell is mapped. Each one is the best answer to a specific question, not the best answer to every question. I once spent three months trying to reproduce a published C. elegans RNAi knockdown result before realizing the original paper used N2 wild-type from a specific stock center. My lab line had drifted genetically over roughly twelve years of routine culture. Phenotype was slightly different, RNAi sensitivity was altered, and the published effect size was completely unreliable against my strain. I went back to a fresh frozen stock, outcrossed once, and the protocol worked as described within a week.
Picking The Right Organism For Your Actual Question
Beginners often start with the most famous model organism and work backward to find a question it can answer. That direction produces messy data. Start with the question, then select the organism that lets you measure what matters. If you need real-time imaging of cell division in a whole multicellular context, zebrafish embryos give you transparency and rapid development. If you need a fully sequenced genome with known gene function and you are studying plant stress responses, Arabidopsis is the direct route. If you are mapping neural circuits in a compact nervous system, C. elegans remains hard to beat for connectivity data. Drosophila covers behavior, development, and genetics exceptionally well. Mice remain necessary when you need mammalian physiology, immune complexity, or translational relevance that flies and worms cannot provide. The tradeoff is cost, space, and time.
Get the Full Details
What People Miss About Maintaining a Model System
Maintenance is not just feeding and storing samples. Genetic drift, microbial contamination, epigenetic accumulation, and lab-specific adaptation all change what your organism actually is over months or years. These changes are invisible unless you monitor them deliberately. I recommend keeping a strain log with passage number, freeze date, mycoplasma or bacterial screen results, and any observed phenotype shifts. Standard practice often skips this entirely. Skipping it creates the exact reproducibility problems that dominate current literature complaints. When working with Drosophila, vial density matters more than most people admit. Overcrowded plates change developmental timing, body size, and stress response profiles. A density difference that looks minor can shift your data enough to create a false positive in a quantitative trait study.
Designing Experiments Around the Model's Actual Limits
Model organisms have well-known blind spots. No single system covers everything. Mice lack the genetic tractability of flies for rapid forward screens. Plants cannot model vertebrate neural function. Worms do not have adaptive immunity. Fish embryos are not miniature adult humans. When I designed a study comparing immune responses across models, I initially planned to use C. elegans as a stand-in for innate immunity screening before moving to mice. The preliminary data showed that key signaling nodes simply do not exist in the same form in nematodes. The pathway appeared conserved on paper but not in functional readouts. Switching to Drosophila as the intermediate model saved months of wasted work and pointed directly at the evolutionary divergence I needed to account for. Counterscreens matter. Always include a negative control that isolates the variable you think is driving the result. Without one, you cannot tell whether your phenotype comes from your manipulation or from standard lab stress, temperature fluctuation, or minor diet changes.
Practical Workflow for a New Model System Project
Step one is defining the exact phenotypic readout before ordering anything. Vague endpoints produce vague data. Step two is sourcing a certified, recently validated strain from a recognized repository. Do not accept an old lab stock without checking its history. Step three is running a baseline characterization under your actual lab conditions. Growth curves, lifespan, baseline gene expression, or whatever matches your readout. This takes one to two weeks depending on the organism and usually reveals condition-specific quirks that published protocols ignore. Step four is pilot experiments with small sample sizes to nail timing, dosing, or induction windows. Step five is the full experiment once the pilot stabilizes. Rushing past step four is the most common reason projects fail quietly.
When a Model System Fails Completely
Sometimes the organism simply cannot answer the question. This happens more often than people admit. I have seen labs push zebrafish into toxicology studies where mammalian metabolic pathways are the actual variable of interest. The fish cleared the compound through routes that do not exist in humans, producing clean data that was biologically irrelevant for the stated goal. In those cases, the correct move is switching systems or adding a complementary model. Two model organisms working in parallel often outperform one model organism pushed beyond its relevance window. Alternative approaches exist when the classic models break down. Organoids, single-organism microfluidic systems, and emerging non-traditional models like planarians or specific nematode species outside C. elegans fill gaps that standard systems leave open. None of these replacements are better across the board. They are better for narrower questions.
The practical reality is that a model system in biology works when you respect its boundaries. It fails when you treat it as a universal proxy. Most bad data comes from the latter mistake, not from flawed techniques.