Why Your Biology Textbook Got This Almost Right
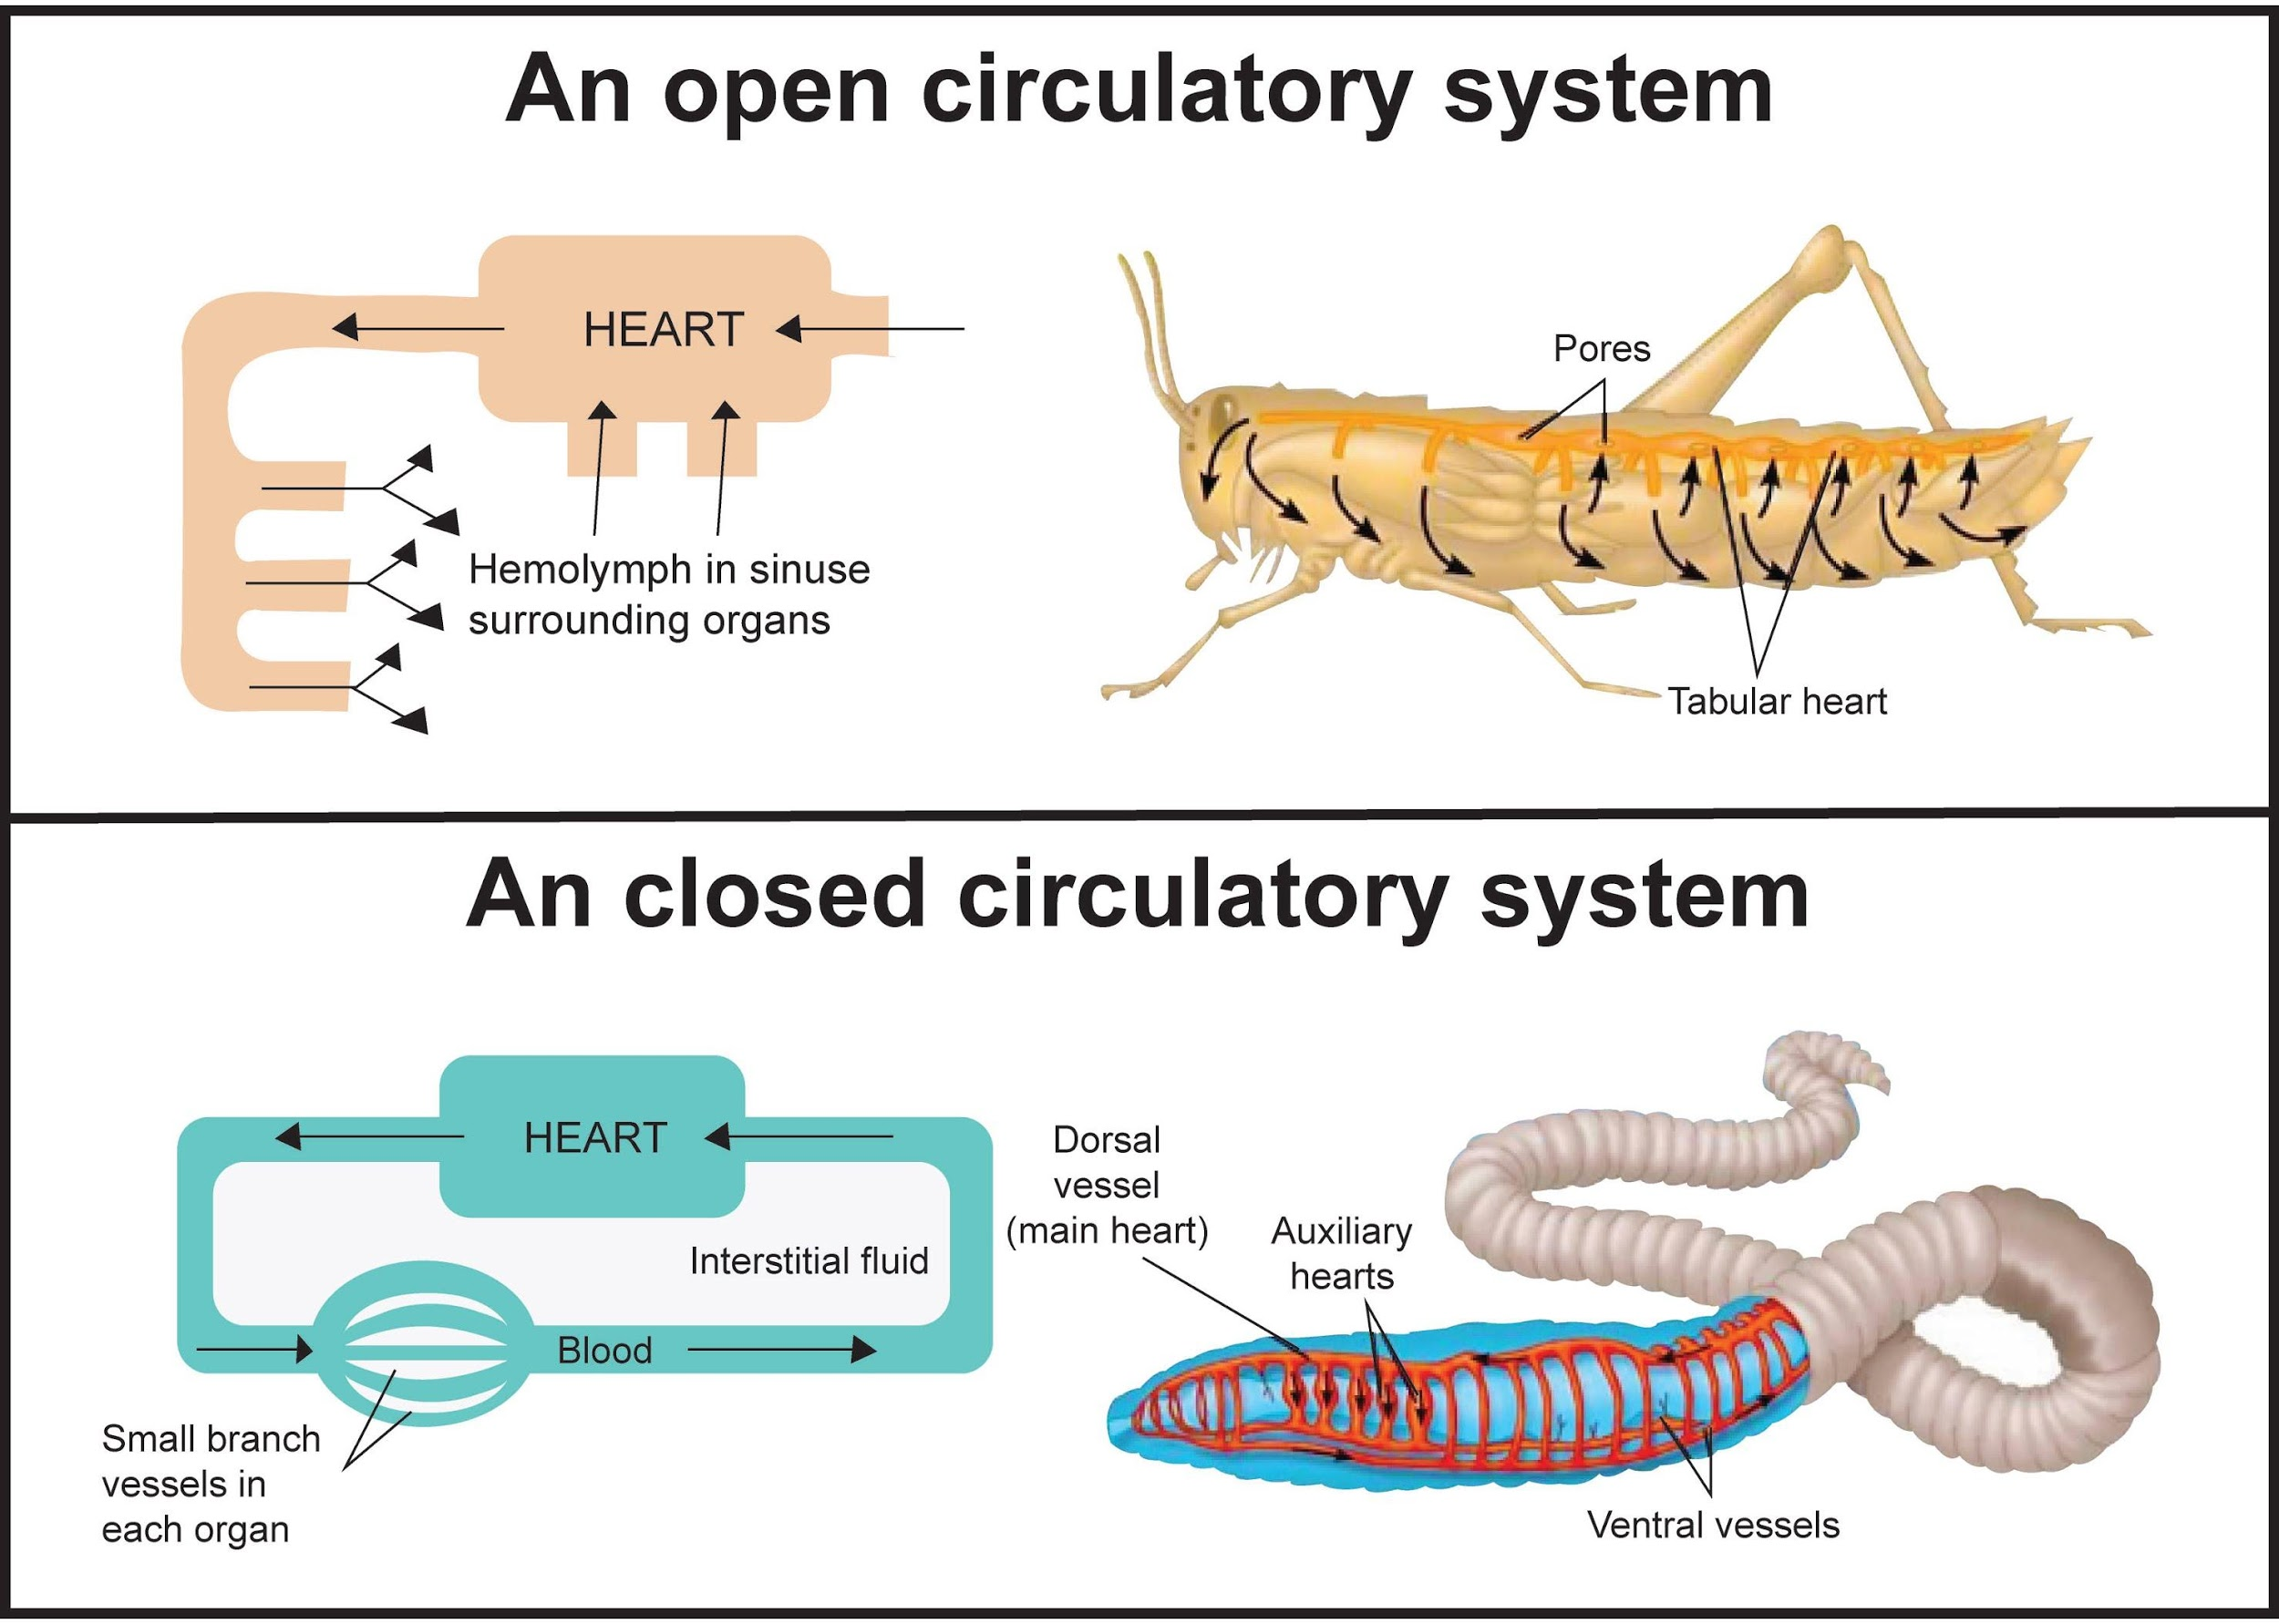
The difference between open and closed circulatory systems comes down to one thing: where the fluid goes after it leaves the pump. In a closed system, blood stays inside vessels the entire time. In an open system, it spills out into cavities and bathes organs directly. That's the textbook version. The actual biology is messier than that, and most people miss the part that matters for understanding how these systems scale with body size. I spent three semesters undergrad dissecting earthworms and squid, and one thing kept coming up in lab reports that students consistently botched. They'd describe the pericardial sinus in an earthworm as an "open space" without explaining why that matters for oxygen delivery under stress. The earthworm's five pseudo-heart structures can constrict independently, which means when the worm burrows into compacted soil, it can shunt blood away from the crop and toward the nerve cord. That's a closed system doing something that looks open from the outside. The septal vessels remain enclosed, but the dorsal and ventral vessels connect through lateral capillaries that function more like channels than true capillary beds. Confusing, right? It should be. Nature doesn't care about clean categories.
Open Vs Closed Circulatory System: The Practical Differences
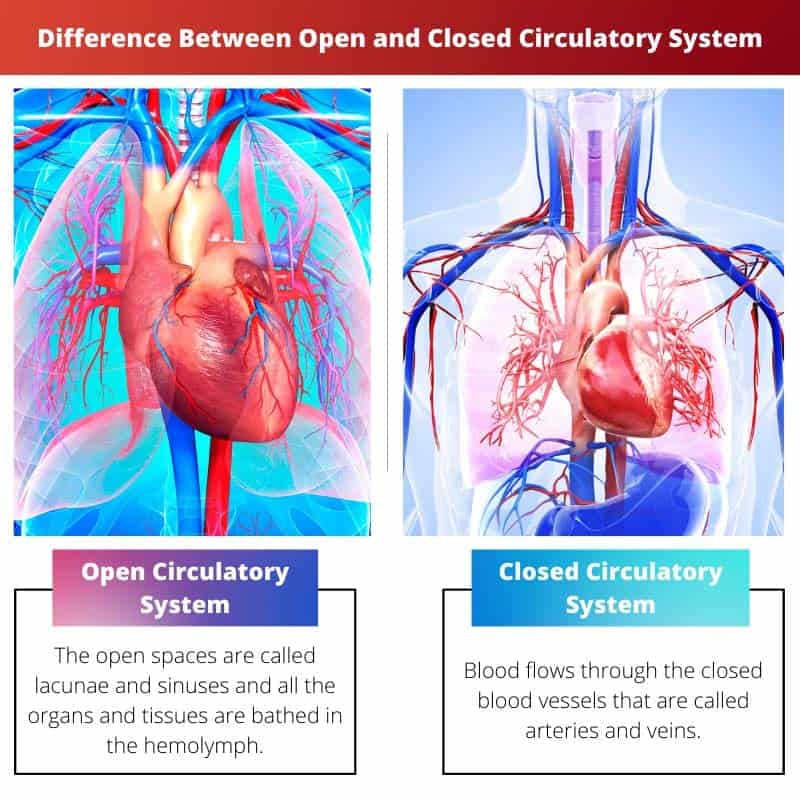
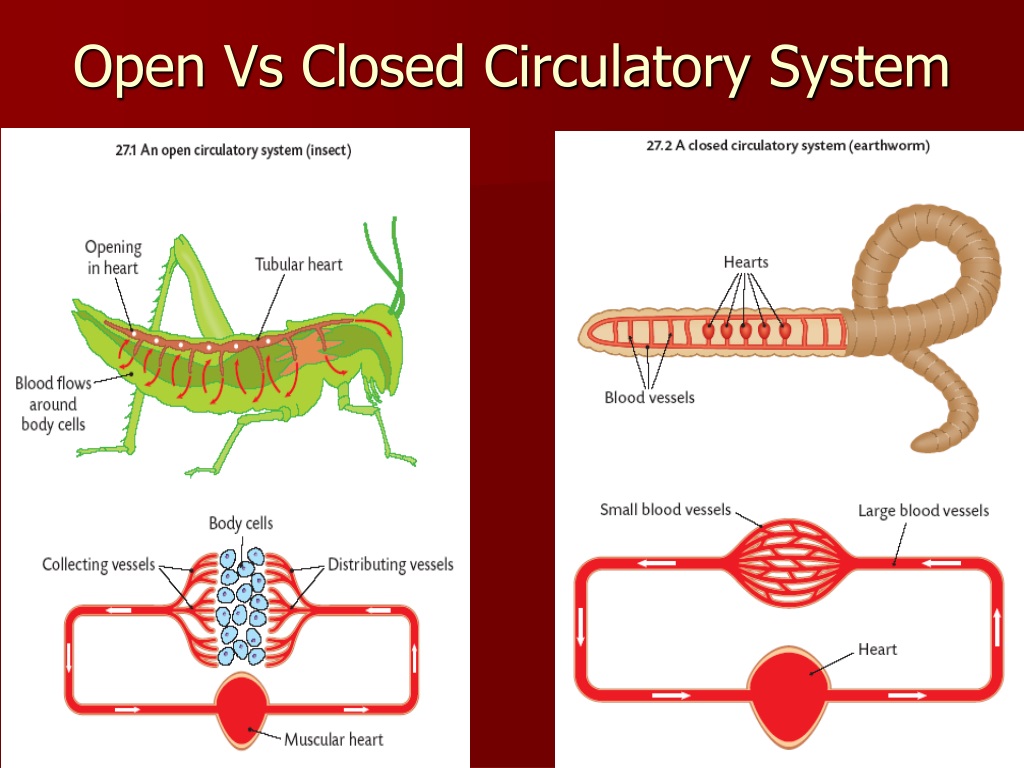
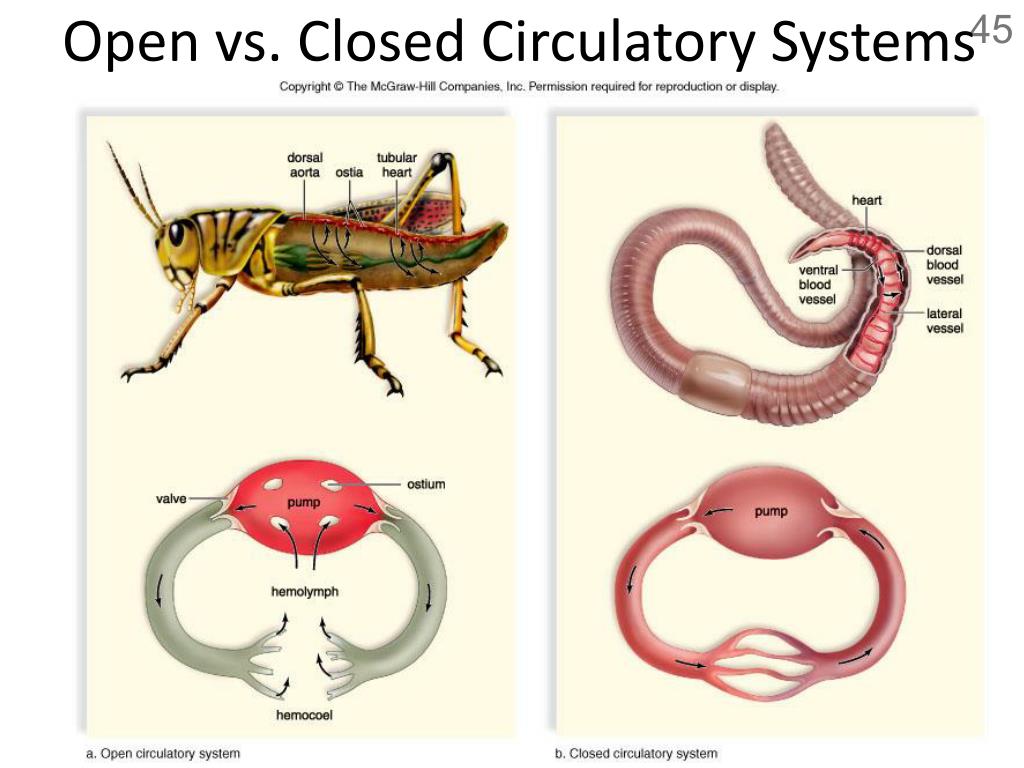
A closed circulatory system keeps blood contained within a continuous network of arteries, veins, and capillaries. The heart pumps blood at relatively high pressure. Blood velocity in mammalian aortas hits about 0.5 meters per second during systole. That pressure drops across the arterioles, which are the primary site of resistance, and by the time blood reaches the venules it's barely moving at all. The exchange surface is the capillary bed, where individual red blood cells slow to approximately 1 millimeter per second to allow gas diffusion. This design supports high metabolic rates because the system can direct flow precisely where it's needed through vasodilation and vasoconstriction. An open circulatory system has a heart that pumps hemolymph into one or more large vessels that terminate in open spaces called sinuses or hemocoels. The fluid then percolates around the organs before re-entering the heart through openings called ostia. Pressure is low, maybe 5 to 20 millimeters of mercury in most arthropods. Flow is slow and largely driven by body movement rather than cardiac output alone. Many insects rely on abdominal pumping and skeletal muscle contractions to move hemolymph, not just the dorsal vessel heartbeat. The key operational difference shows up under demand. When a vertebrate runs, the sympathetic nervous system can increase cardiac output by a factor of four to five while simultaneously redirecting blood from the gut to the muscles. An octopus can do something similar through its three hearts, but a grasshopper can't really do anything comparable. If you restrain an insect's legs and abdomen, its hemolymph flow drops significantly because the accessory pulsatile organs in the legs and wings stop contributing to circulation. That's why pinned specimens in a dissection tray look perfectly fine one minute and then start showing signs of stagnation the next. Not because they're dying from the dissection, but because you've removed their primary circulation mechanism.
Here's something most introductory courses skip. The distinction isn't binary. Some organisms sit in a gray zone that makes classification annoying. Crustaceans like crabs have a closed branchial heart system where blood flows through gill capillaries in a truly closed loop, but then empties into an open hemocoel for the rest of the body. So a crab has both a closed subsystem and an open system operating in series. If you're writing a paper and need to label the whole thing, you'd call it open, but that label hides the fact that gas exchange happens under closed conditions at higher pressure, which is actually more efficient than what land insects do with their tracheal systems. I ran into a real problem during a comparative physiology project where I was measuring hemolymph protein concentrations across twelve species of decapod crustacean. The literature value for port crab hemolymph osmolarity was listed as about 1000 milliosmoles, but my refractometer readings came back consistently 80 milliosmoles lower. I spent two weeks tracking down the discrepancy before I realized the published values were measured from the sinus venosus of anaesthetized animals, while I was sampling from the pericardial sinus of restrained but conscious specimens. The stress response in crustaceans causes a rapid shift of water from the hemolymph into the gut lumen and excretory organs, concentrating the remaining fluid. The ostia have sphincter-like valves that close under stress to prevent backflow, which temporarily isolates the pericardial sinus and creates a micro-compartment with different composition than the general hemocoel. I had to switch to anaesthetized sampling to match the published data, but even then, the values varied by season and molting stage. Post-molt crabs have hemolymph volumes that can be 15 percent higher than intermolt animals, and the protein concentration drops proportionally because the new exoskeleton hasn't been hardened yet. That's the kind of detail that doesn't make it into the summary tables.
Get the Full Details
Where Each System Wins and Where It Fails
Closed systems support larger body sizes and higher activity levels. That's not a debate. The pressure differential you can maintain across a continuous vascular network allows for rapid, targeted delivery of oxygen and nutrients. Mammals and birds push this to the extreme with four-chambered hearts and complete separation of oxygenated and deoxygenated blood, achieving cardiac outputs around 5 liters per minute at rest and up to 25 liters per minute in endurance athletes. The capillary density in mammalian skeletal muscle is roughly 300 to 400 capillaries per square millimeter, which gives a diffusion distance of about 10 to 20 micrometers from any cell to a capillary. That's tight enough for aerobic metabolism to sustain high rates of ATP production. Open systems work fine for small, slow organisms. Insects are the poster children, and they got here by solving the oxygen delivery problem differently. Most insect hemolymph doesn't carry oxygen at all. The tracheal system delivers O2 directly to tissues through a network of air-filled tubes. Hemolymph's job is mostly nutrient transport, waste removal, and hydrostatic pressure for movement. The circulatory system in insects is almost secondary to respiration. You could argue the insect circulatory system is underqualified for what it's asked to do, but it works because the animal doesn't need it to carry oxygen. If you tried to replace an insect's tracheal system with a closed circulatory oxygen transport system, you'd need something like ten times the heart output just to move equivalent amounts of O2, and the energy cost would be unsustainable at the insect's size range. The limitation of open systems becomes obvious when you look at size constraints. The largest insects today are maybe 15 to 20 centimeters in wingspan. The largest known insects from the Carboniferous period, like Meganeura, had wingspans approaching 70 centimeters, and the leading hypothesis for that size ceiling is atmospheric oxygen concentration. Higher O2 partial pressure allows diffusion through tracheae to reach further into tissues. When oxygen levels drop, open circulatory systems paired with tracheal respiration can't support large bodies because the hemolymph can't generate enough pressure to push fluid through narrow exchange spaces fast enough. Earthworms, which use a closed system and breathe through their skin, can grow to over 3 meters in the case of Driloleirus macroleiotos, the giant Oregon earthworm. Skin breathing only works at that scale because the closed system keeps the fluid moving efficiently enough to support a larger volume of metabolically active tissue.
The main tradeoff is energy versus control. Open systems run at low pressure and consume far less energy. A resting cockroach uses about 0.1 milliliters of oxygen per gram per hour. A mouse of similar mass uses roughly 1.5 milliliters per gram per hour. The cockroach's circulatory system doesn't need to generate much pressure because its metabolic demand is low and its delivery method is passive diffusion through tracheae. But that low demand also means the cockroach can't sustain prolonged high activity. Take away the tracheal shortcut and an insect with an open system couldn't keep up with a vertebrate of comparable size in any endurance test. Another nuance that gets glossed over: the role of the heart itself. In vertebrates, the heart is a single centralized pump. In insects, the dorsal vessel is often described as a simple tube heart, but in many species it's divided into a posterior pumping chamber and an anterior aorta, with additional auxiliary pulsatile organs in the wings, legs, and abdomen. These accessory pumps can operate independently and are often more important for circulation than the dorsal vessel itself during normal activity. I learned this the hard way when I was trying to record hemolymph flow velocity in cockroaches using fluorescent microbeads. The dorsal vessel contraction rate was about 100 beats per minute, but the beads moved in bursts that didn't correlate with the dorsal vessel at all. It took someone in the lab pointing out that the anterior leg pulsatile organ was firing at a different phase to make sense of the data. The main heart wasn't the dominant driver. The accessory organs were, and they were responding to leg movement, not a central rhythm. If you're studying this for a class or trying to apply the concepts somewhere, don't fall into the trap of thinking closed is always superior. It's superior for high-metabolism, large-bodied, active organisms. For small, low-metabolism, or externally respiring organisms, open is perfectly adequate and energetically cheaper. The evolutionary trajectory isn't a ladder from open to closed. It's a set of solutions to different problems. Arthropods evolved open systems and then solved the oxygen problem with tracheae. Vertebrates evolved closed systems and kept using blood for gas transport. Both approaches produced successful lineages. The fact that humans and squids both have something we loosely call a heart doesn't mean they're doing the same thing. A squid has three hearts because two of them are branchial hearts that pump blood through the gills independently of the systemic heart. If one branchial heart fails, the gill on that side stops receiving blood, but the animal doesn't immediately die. In a mammal, if one ventricle fails, everything stops within minutes. Different failure modes, different design philosophies.