The actual outputs from your cells right now
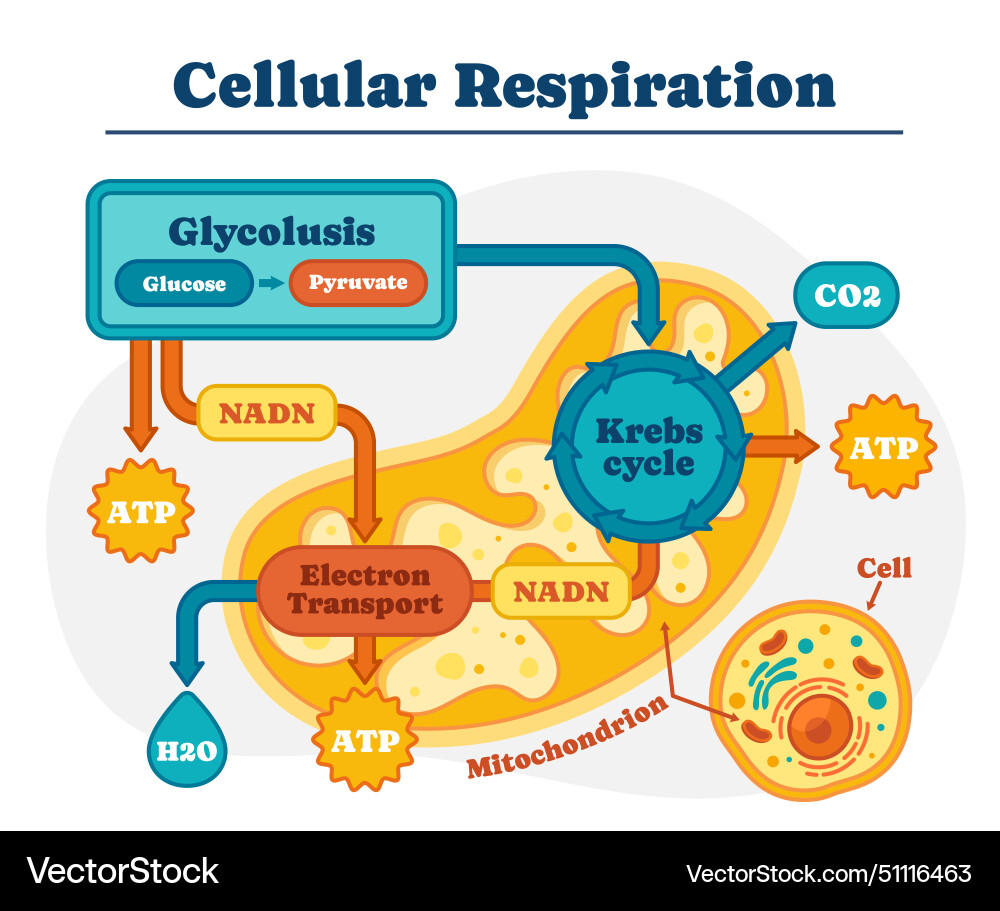
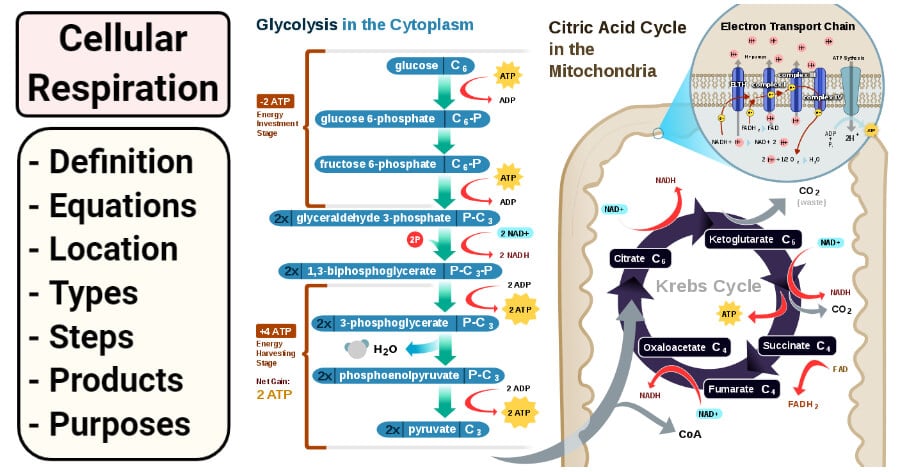
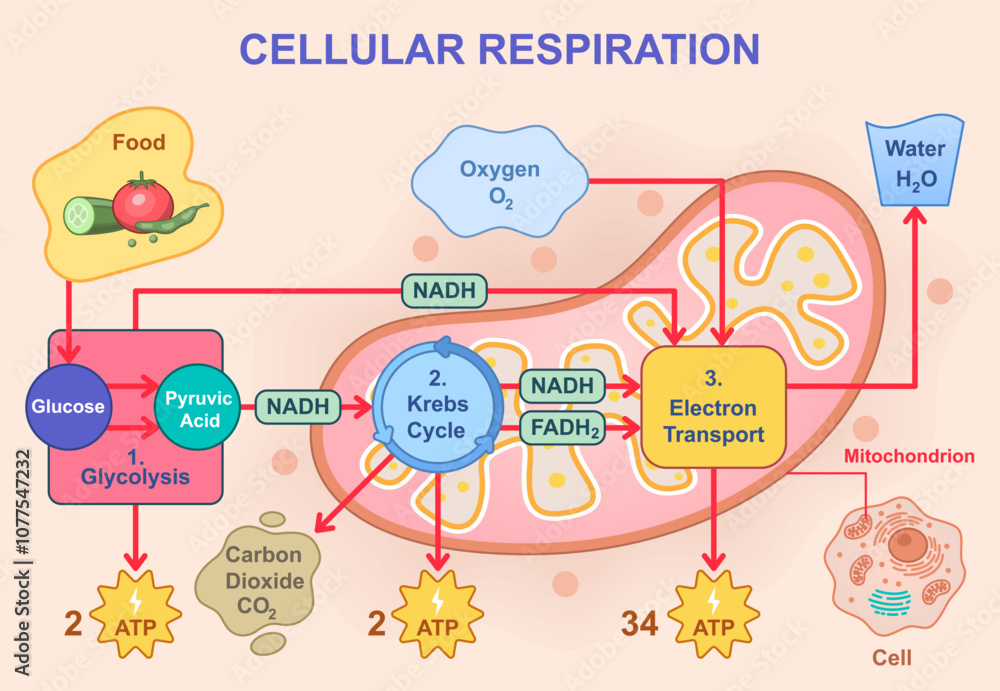
Cellular respiration is the process where cells break down glucose and other fuel molecules to produce ATP. The overall equation is straightforward: C6H12O6 + 6O2 6CO2 + 6H2O + ATP. Those are the three main Products Of Cellular Respiration. Carbon dioxide, water, and adenosine triphosphate. That's it. Everything else is just the mechanism. But here's where most textbooks oversimplify things. The ATP yield isn't a fixed number. Older sources will tell you 36 or 38 ATP per glucose molecule. Modern biochemistry puts it closer to 30 to 32. The difference comes down to proton leak across the inner mitochondrial membrane and the cost of shuttling NADH from the cytoplasm into the mitochondria. The malate-aspartate shuttle is more efficient than the glycerol-3-phosphate shuttle, and which one your cells use depends on the tissue type. Heart and liver prefer the malate-aspartate route. Skeletal muscle and brain tend to use the glycerol-3-phosphate version, which costs you roughly two ATP per glucose. I ran into this exact discrepancy a few years ago while debugging why an energy expenditure model I was building kept overestimating basal metabolic rate by about eight percent. The model was hardcoded to 38 ATP per glucose. Once I switched it to the 30-to-32 range and factored in tissue-specific shuttle usage, the output aligned with measured VO2 data. Took me about two days to track down because every introductory resource I checked had the old number.
Products Of Cellular Respiration in different conditions
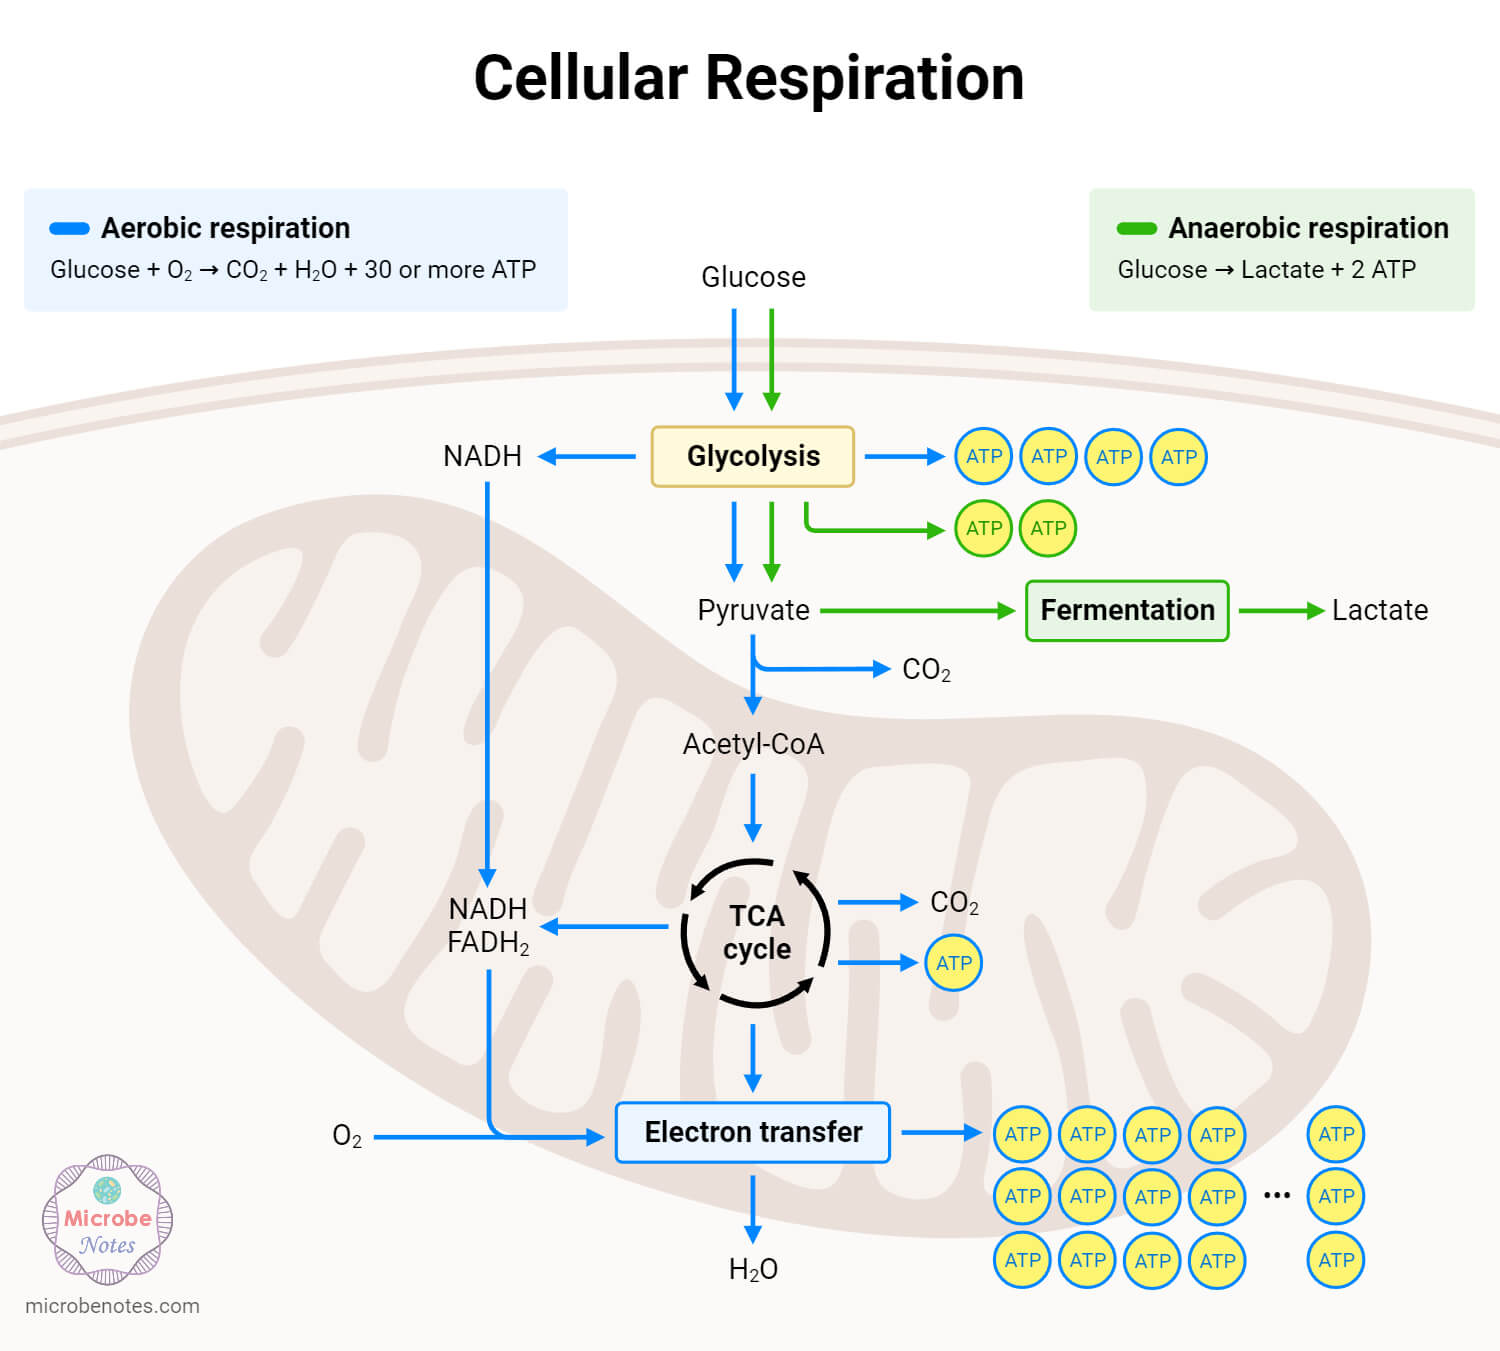
The equation I wrote above assumes aerobic conditions. That means oxygen is present and the electron transport chain can function. When oxygen runs out, the whole system changes. The Products Of Cellular Respiration under anaerobic conditions are completely different, and they vary depending on the organism. In human muscle cells during intense exercise, for instance, pyruvate gets converted to lactate. You get two ATP per glucose from glycolysis alone. No citric acid cycle. No oxidative phosphorylation. The NAD+ has to be regenerated some other way, and lactate dehydrogenase handles that. This is why your muscles burn during a sprint. Lactate accumulation drops the pH inside the cell. It's not the lactate itself causing fatigue, but the accompanying hydrogen ions interfering with calcium handling in the sarcoplasmic reticulum and reducing actin-myosin binding affinity. That's a separate issue, but it matters for anyone actually studying exercise physiology instead of just memorizing the fermentation equation. In yeast and some bacteria, you get ethanol and carbon dioxide instead of lactate. That's alcoholic fermentation. Two ATP per glucose, same as lactic acid fermentation. The pathways diverge after pyruvate. Pyruvate decarboxylase removes CO2 to form acetaldehyde, then alcohol dehydrogenase reduces it to ethanol using NADH. Again, the point is regenerating NAD+, not producing useful energy. The ethanol is waste.
Here's something most people miss: the water produced in cellular respiration isn't just H2O floating around. It's formed at complex IV of the electron transport chain when molecular oxygen accepts four electrons and four protons to become two water molecules. One glucose molecule yields about six water molecules through this process. In desert rodents like the kangaroo rat, water from cellular respiration is actually significant for survival. They can live their entire lives without drinking free water because the water produced internally from oxidizing food molecules covers their needs. Their kidneys are adapted to concentrate urine far beyond what humans can manage, minimizing water loss. This isn't a minor footnote. It's a core adaptation.
Get the Full Details
What actually gets used and what gets discarded
ATP is the useful product. The cell uses it immediately for mechanical work, transport work, and chemical work. It doesn't store ATP in any meaningful quantity. A typical cell holds only enough ATP for a few seconds of activity. That's why the turnover rate is so high—your body recycles its own body weight in ATP every day. The carbon dioxide is a waste product that diffuses into the blood, travels to the lungs, and gets exhaled. The water stays in the cell or enters the extracellular fluid. Both CO2 and H2O can be reabsorbed or reused in other pathways, but in the context of respiration itself, they're end products. The intermediate molecules matter too. NADH and FADH2 are produced during glycolysis, the link reaction, and the citric acid cycle. They carry electrons to the electron transport chain. They aren't final products. They're electron carriers that get reoxidized back to NAD+ and FAD. If you're tracking the complete flow, you need to account for them as transient intermediates, not outputs. One practical issue that comes up in lab settings: when you're measuring respiration rates with a respirometer, you have to account for the CO2 being absorbed. If you're using potassium hydroxide or soda lime to soak up the carbon dioxide, the volume change you measure reflects only oxygen consumption. If you forget the CO2 absorber, your readings will be wrong because the CO2 produced partially offsets the volume decrease from oxygen use. I've seen this mess up undergraduate lab results more times than I can count. The students either skip the absorber step or use exhausted absorbent material that can no longer capture CO2 effectively. Either way, the calculated respiratory quotient ends up inaccurate, and the whole exercise becomes pointless.
Another edge case: the P/O ratio. This is the number of ATP molecules produced per oxygen atom consumed. It's not constant. Complex I pumps more protons than complex III or IV individually, but the overall stoichiometry depends on the H+/ATP ratio of ATP synthase, which varies between organisms. In mammals, it's roughly 4 protons per ATP. The theoretical maximum P/O ratio for NADH is about 2.5, and for FADH2 it's about 1.5. These are averages. Actual values in living cells can deviate due to proton leak, uncoupling proteins, and variations in membrane composition. Uncoupling protein 1 in brown adipose tissue is a deliberate example of this—protons flow back across the membrane without making ATP, and the energy is released as heat instead. This is how hibernating animals and newborns generate warmth. The Products Of Cellular Respiration in that case include heat as a significant output, not just ATP, CO2, and water.
Common misconceptions that waste time
People often think cellular respiration only happens in mitochondria. Glycolysis occurs in the cytoplasm. The link reaction and citric acid cycle are in the mitochondrial matrix. Oxidative phosphorylation happens at the inner mitochondrial membrane. All three stages are part of cellular respiration, and they're spatially separated. Don't conflate them. Another one: ATP is not the only energy currency. GTP is produced directly in the citric acid cycle when succinyl-CoA is converted to succinate. It's functionally equivalent to ATP and can be used by the same enzymes after a nucleoside-diphosphate kinase reaction converts it. Some cells use GTP specifically for protein synthesis initiation. It's a small detail but worth knowing if you're reading primary literature on translation. The process also doesn't just use glucose. Fatty acids enter through beta-oxidation, producing acetyl-CoA that feeds directly into the citric acid cycle. Amino acids can be deaminated and converted to intermediates at various points—pyruvate, acetyl-CoA, or citric acid cycle intermediates like alpha-ketoglutarate or oxaloacetate. The Products Of Cellular Respiration remain the same regardless of the starting fuel, but the ATP yield per gram differs significantly. Fats produce roughly twice the ATP per gram compared to carbohydrates because they're more reduced. This is why endurance athletes rely on fat oxidation for prolonged effort.

If you're studying this for an exam, focus on understanding the flow of carbon and electrons rather than memorizing every enzyme name. The carbon atoms from glucose end up in CO2. The electrons end up reducing oxygen to water. The energy released during electron transfer drives proton pumping, and the proton gradient drives ATP synthesis. That's the core logic. Everything else is detail. There's no single software tool or download that will teach you this better than working through the pathways on paper. What helps is drawing the connections between the stages and tracking one glucose molecule through every step. You'll see where the ATP comes from, where the CO2 is released, and where the water forms. The picture becomes clearer once you stop treating each stage as a separate topic and start seeing it as one continuous process with inputs, outputs, and energy transformations at every step.