Setting Up a Cross Without Losing Your Mind
A Punnett square is just a grid where you lay out the possible gametes from each parent along the top and side, then fill in the boxes by combining them. That's basically it. The problem isn't the tool itself. It's that most practice problems are written in ways that make the tool look more complicated than it actually is, and when students hit anything beyond simple monohybrid crosses, things fall apart fast. I've been grading these things and helping people through them for long enough that I can spot the exact moment someone's about to get confused. It usually happens at the dihybrid stage. Here's what I tell people to do instead of starting with a 4x4 grid blindly.
Punnett Square Practice Problems
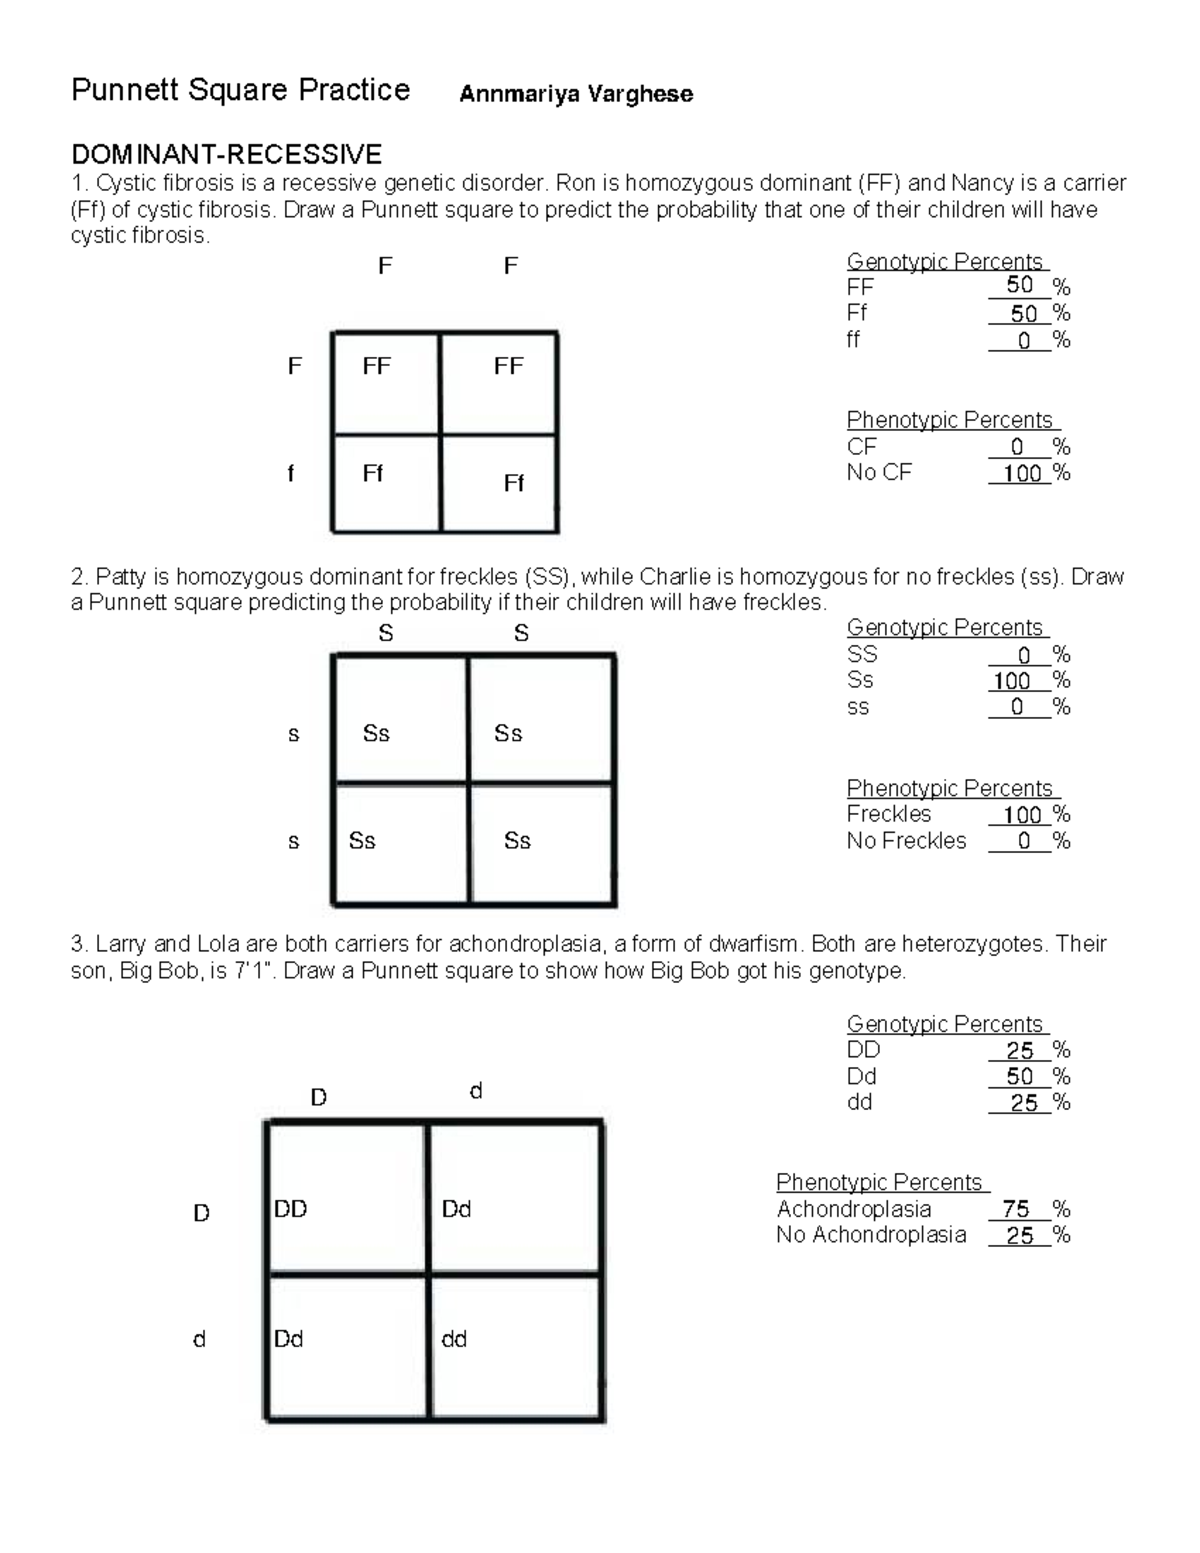
The standard way to work through these problems is to first figure out what alleles each parent can produce. If you're dealing with a single gene, like flower color where purple (P) is dominant over white (p), and you're crossing two heterozygotes, each parent produces P and p gametes. You put one set across the top, the other set down the side, and fill in. P | p P -- PP | Pp
p -- Pp | pp The phenotypic ratio comes out to 3 purple : 1 white. That's textbook. But here's where people start making mistakes that cascade through every problem after this one.
Get the Full Details

Where Most People Go Wrong
The biggest issue I see is treating Punnett squares as if they're probability calculators rather than what they actually are: a visual enumeration tool. They don't replace the product rule or sum rule. They just organize the same math in a grid. When someone asks for the probability of getting at least one dominant allele from that cross, they shouldn't be counting boxes. They should be applying basic probability. The answer is 3/4. Counting boxes gives you the same result, sure, but it doesn't scale. Another thing that catches people off guard is the assumption that all gamete types are equally likely. This seems obvious until you hit linkage, and that's the first time most students realize their 4x4 grid just gave them a completely wrong picture. I ran into a problem recently where the genes were on the same chromosome about 8 map units apart, and the expected recombinant frequency was roughly 8%. A standard dihybrid Punnett square assumes independent assortment and would give you a 1:1:1:1 gamete ratio instead of something closer to 46% parental types and 4% recombinants each. The grid literally cannot represent this accurately without modifying the numbers inside it. I had to teach someone to put the actual gamete frequencies into the grid boxes instead of assuming equal distribution. Once they saw that, it changed how they approached every linked gene problem after that.
Dihybrid Crosses and the Forked-Line Method
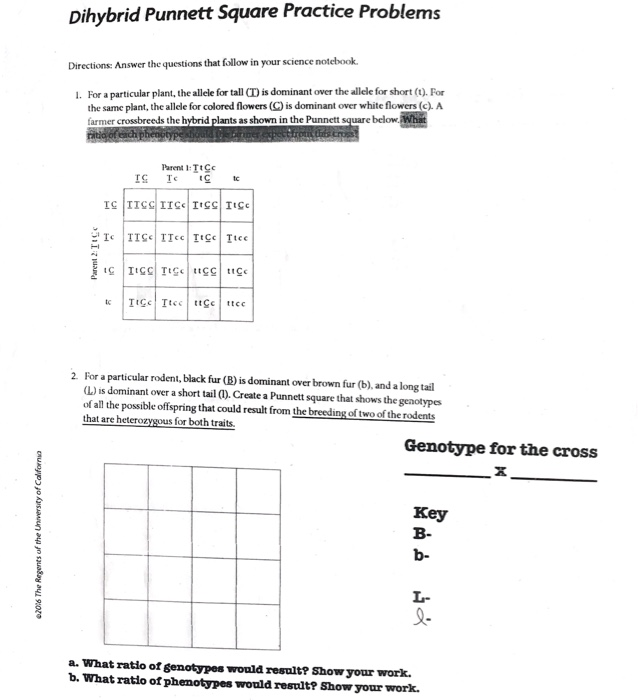
When you move to two genes, the 4x4 grid works, but it's tedious and you have to be very careful about writing out all eight possible gamete combinations correctly. I prefer showing people the forked-line method alongside the square because it reveals something the square obscures. With two independently assorting genes, say AaBb crossed with AaBb, you can analyze each gene separately and then multiply the outcomes. The A gene gives you 3/4 dominant, 1/4 recessive. The B gene gives you the same. Multiply them: 9/16 dominant for both, 3/16 dominant A recessive B, 3/16 recessive A dominant B, 1/16 recessive for both. Same result as the 16-box grid. Takes less time, fewer places to make a transcription error. But here's the nuance nobody emphasizes: this multiplication only works because of independent assortment. As soon as genes are linked, on the same chromosome, or when you have epistasis where one gene masks another, you can't just split them up and multiply. The 9:3:3:1 ratio vanishes. With epistasis, like the classic 9:3:4 recessive epistatic ratio in Labrador retriever coat color, the phenotypic ratios shift entirely while the underlying genotypic probabilities stay calculable. You need to track the genotypes through the square first, then apply the epistatic rule afterward to get phenotypes. Doing it in reverse will give you the wrong answer every time.
Sex-Linked Inheritance
These problems require a slightly different setup because the sexes aren't symmetrical. A cross between a carrier female (X^H X^h) and a normal male (X^H Y) produces four possible offspring combinations, but the ratios differ between males and females. Males get their X from the mother, so there's a 50% chance a son inherits the recessive allele and expresses the trait. Females need two copies, so they're much less likely to be affected. The grid handles this fine if you remember that males only carry one X chromosome and the Y doesn't carry the allele you're tracking. Punnett squares break down when you're dealing with polygenic traits, multiple alleles with more than two variants in a population, or any scenario where the sample space gets large enough that drawing a grid is pointless. For three genes, you'd need an 8x8 grid with 64 boxes. It's not impossible, but it's also not a good use of your time. At that point, the branching probability method is significantly faster and less error-prone. For population-level genetics with multiple alleles and unknown genotypes, you're better off moving straight to Hardy-Weinberg calculations or using a computational tool. There's also the matter of incomplete penetrance and variable expressivity, which Punnett squares simply cannot model. A square will tell you that 25% of offspring should show a recessive phenotype, but if penetrance is 80%, only 20% actually will. The square doesn't know this. It assumes perfect penetrance and complete dominance by default. I've seen students lose points on exams because they didn't account for this distinction, not because they drew the grid wrong, but because they trusted the grid to give them the whole story.
A Practical Walkthrough
Let me walk through a problem that trips up a lot of people. Cross a homozygous dominant tall plant (TT) with a heterozygous tall plant (Tt). Set up the square. Parent one produces only T gametes. Parent two produces T and t gametes. T | T T -- TT | TT
t -- Tt | Tt Every offspring is tall. Genotypically, half are TT and half are Tt. The phenotypic ratio is 100% tall. Simple enough. Now here's a trickier version: what if you're told the offspring show a 1:1 ratio of tall to short? What were the parents? Working backward from the result, a 1:1 ratio means one parent must contribute only the recessive allele and the other must be heterozygous. So the cross is Tt x tt. You can verify this with a square, and it checks out. Half Tt, half tt. Half tall, half short. The skill here isn't drawing the square. It's knowing when the square is the right tool and when it's a crutch you should stop leaning on.