The Mechanism Is Straightforward Until You Actually Look At It
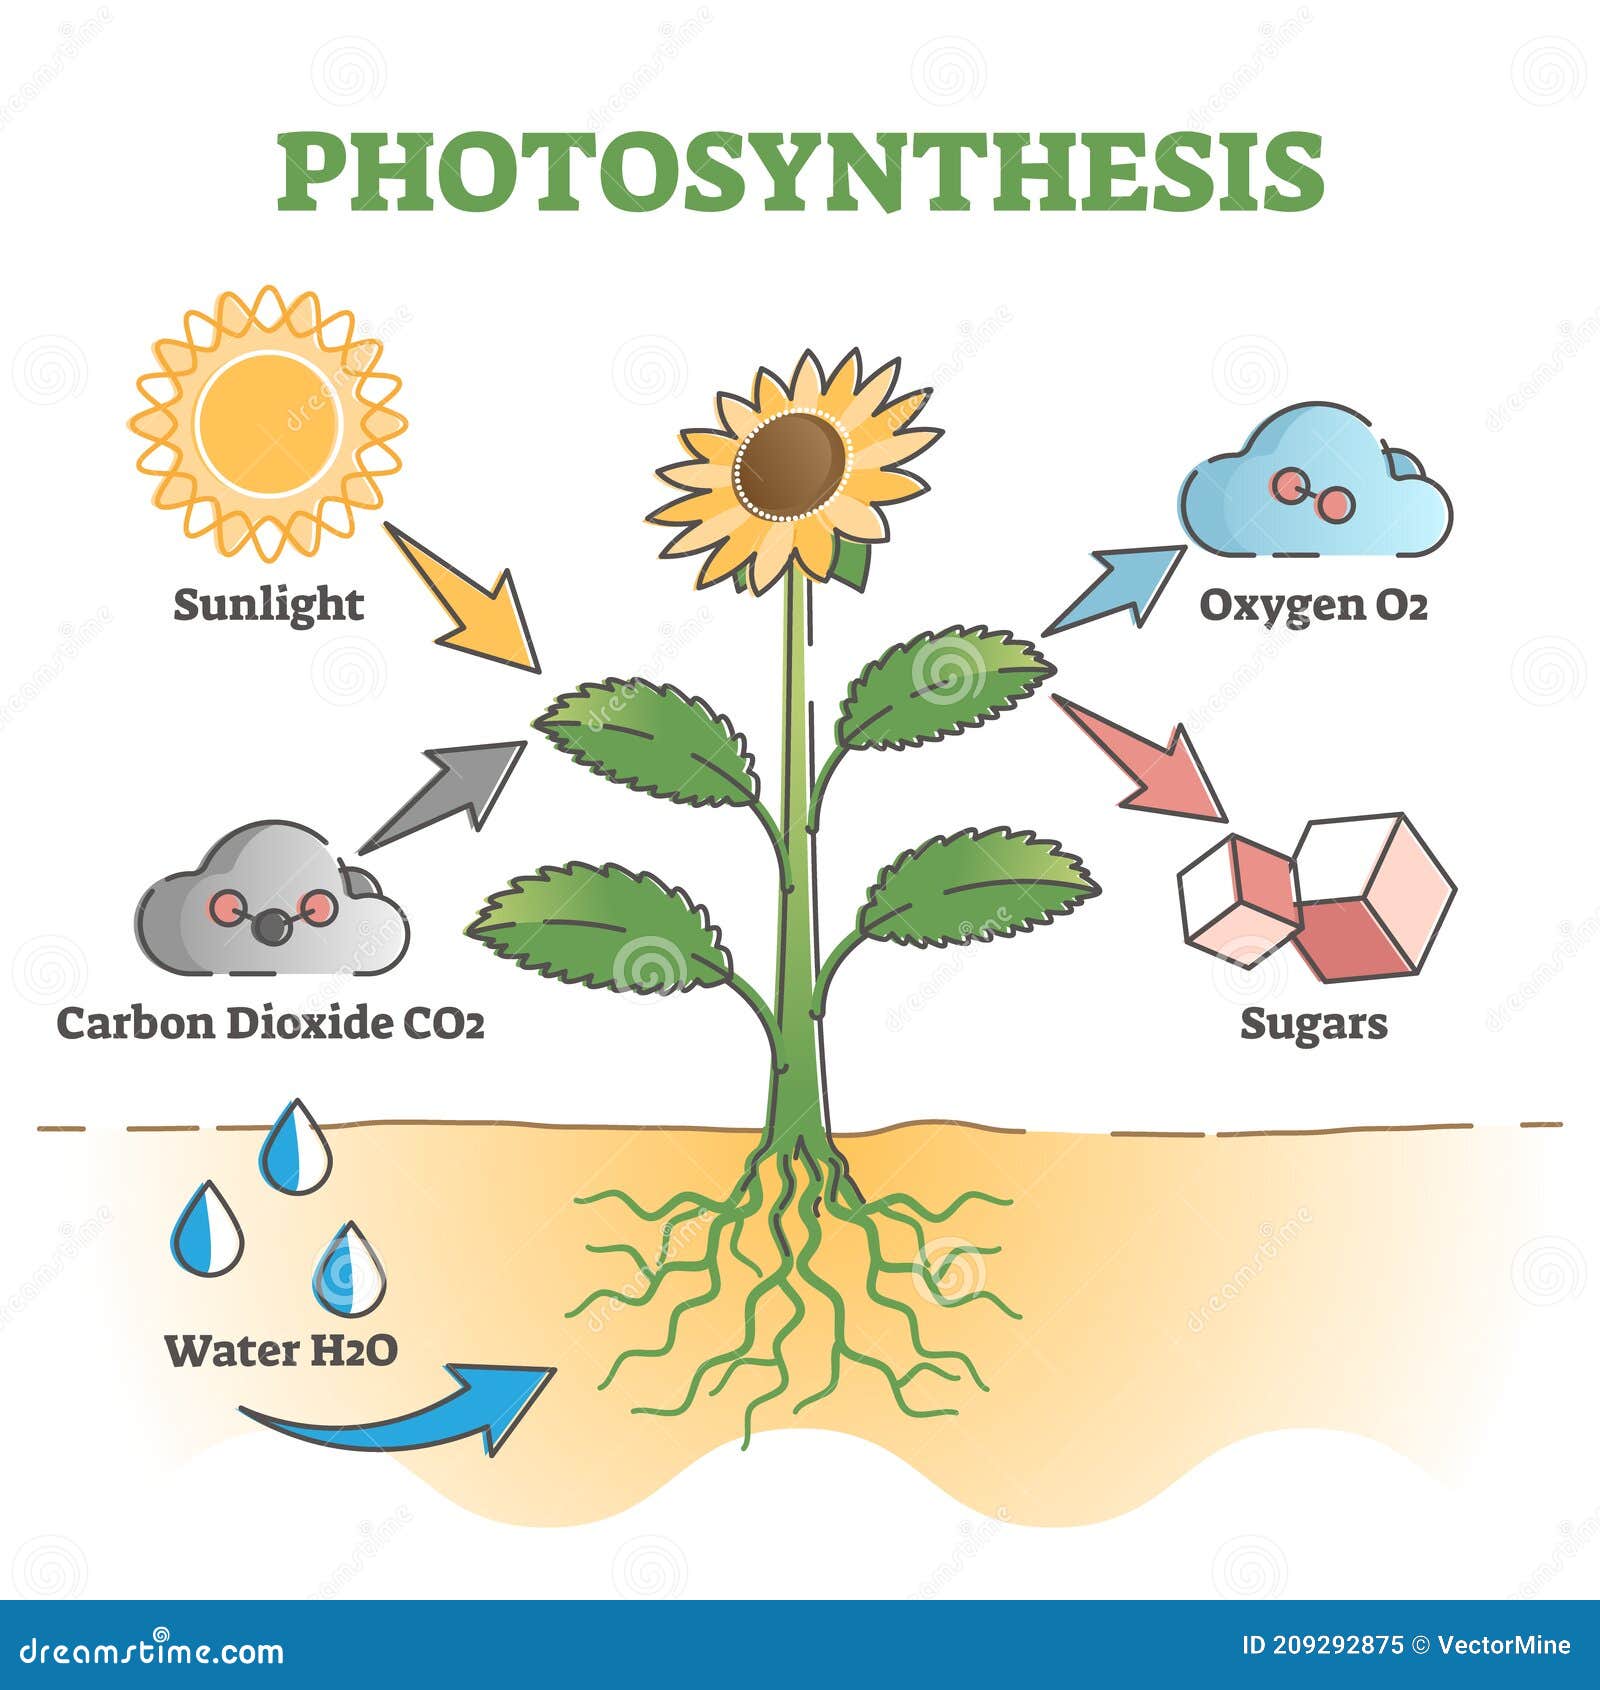
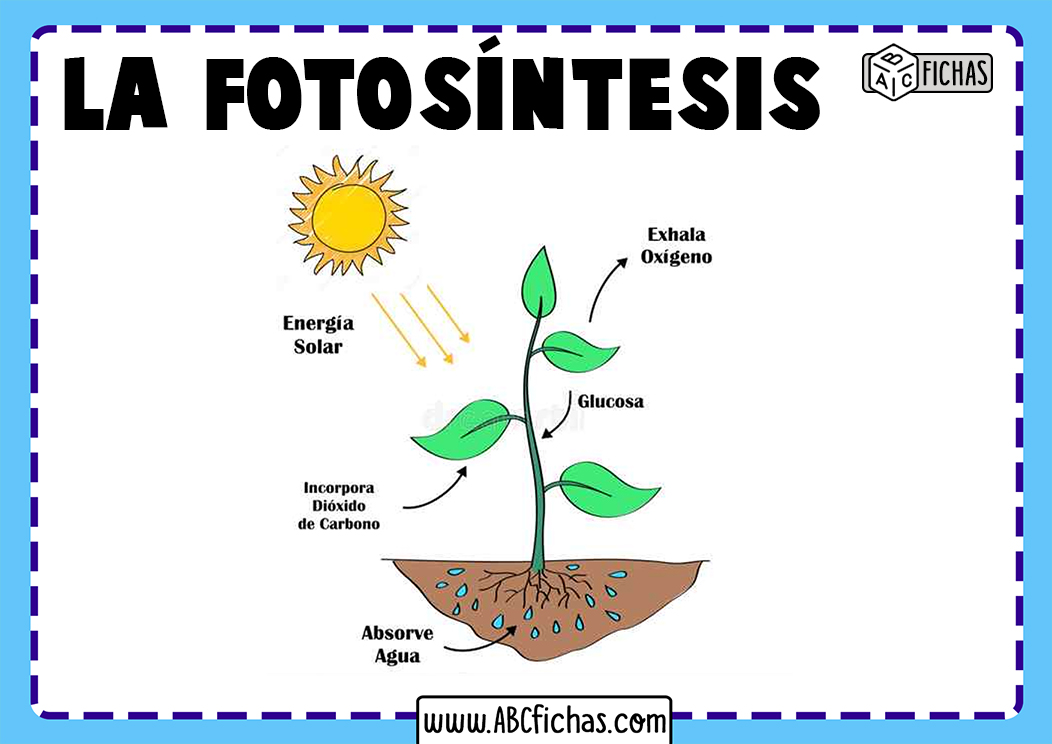
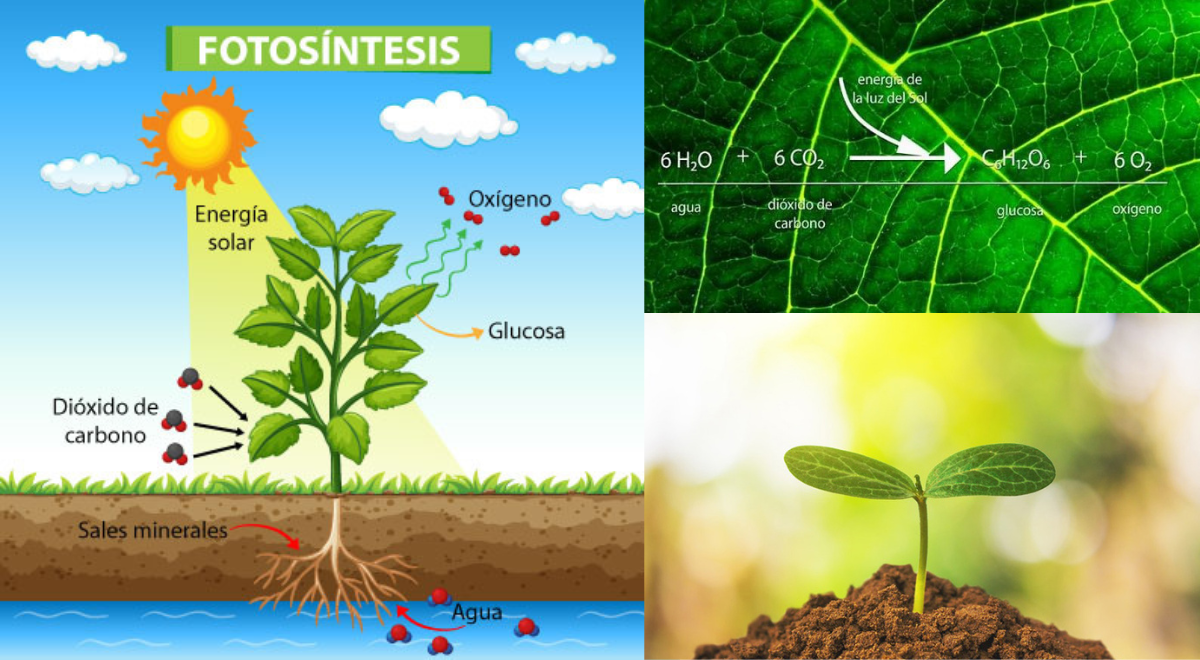
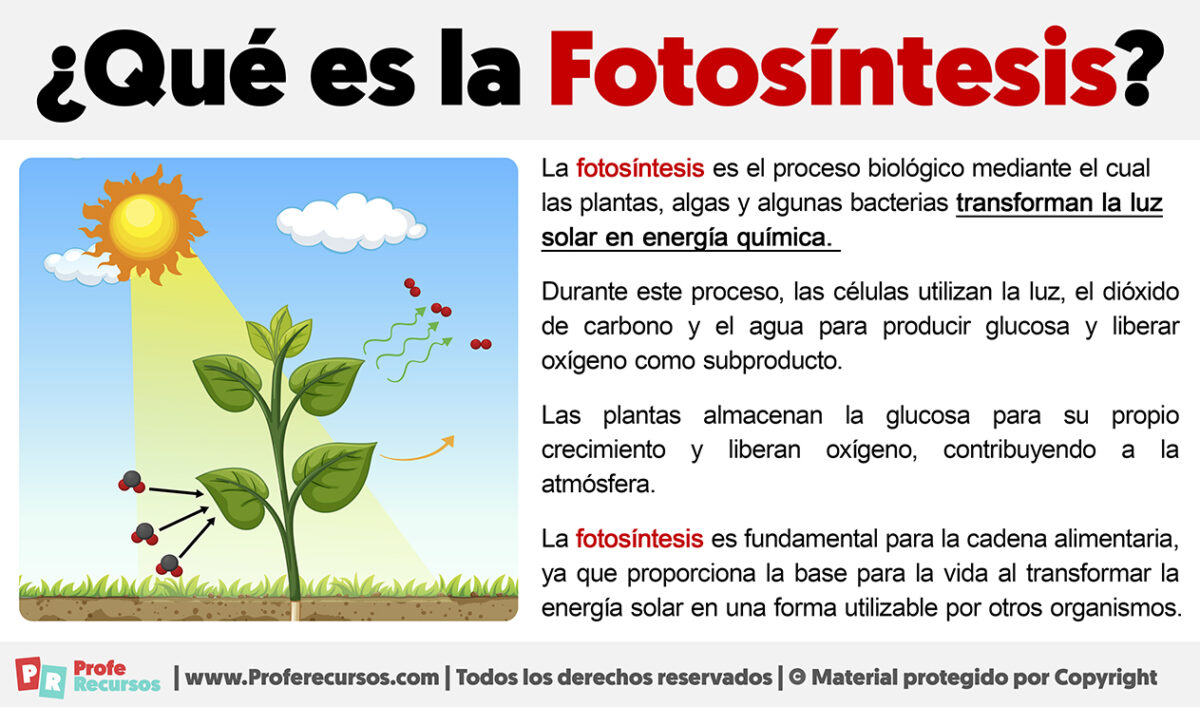
Photosynthesis is the process by which photoautotrophic organisms convert light energy into chemical energy stored in carbohydrate molecules. Plants, algae, and cyanobacteria all use this same general framework. The core equation is simple enough: carbon dioxide and water, in the presence of light, produce glucose and oxygen. But the actual machinery running inside the chloroplast is far messier than that single sentence suggests. The process splits into two distinct phases. The light-dependent reactions happen in the thylakoid membranes. Photosystem II absorbs photons, excites electrons, and splits water molecules as a byproduct, releasing oxygen. Those electrons travel through an electron transport chain, pumping protons into the thylakoid lumen and creating a gradient. ATP synthase uses that gradient to generate ATP. Photosystem I re-energizes the electrons, which ultimately reduce NADP+ to NADPH. Both ATP and NADPH then feed into the Calvin cycle in the stroma, where carbon fixation occurs and sugars are synthesized. I spent a semester monitoring oxygen evolution rates in isolated chloroplast preparations from spinach. The protocol seemed basic enough, but the variables you think don't matter end up breaking everything. One time I noticed inconsistent oxygen readings across replicates, and after ruling out instrument error, I discovered the chloroplast suspension had been sitting under the lab bench light for too long between extraction and measurement. The photosystems had undergone photoinhibition from uncontrolled exposure. The fix was straightforward: keep everything on ice, work in dim green light when possible, and run the assay within twenty minutes of isolation. It cut my variance down significantly.
The Calvin cycle itself involves ribulose-1,5-bisphosphate carboxylase-oxygenase, commonly called Rubisco. This enzyme fixes CO2 onto RuBP, producing two molecules of 3-phosphoglycerate. Through a series of reduction and regeneration steps, some of those carbons leave the cycle as glyceraldehyde-3-phosphate, which the plant converts into glucose and other carbohydrates. The rest regenerate RuBP so the cycle can continue. Here is something most introductory courses gloss over: Rubisco is also an oxygenase. When O2 binds to Rubisco instead of CO2, the plant initiates photorespiration, a process that consumes energy and releases previously fixed carbon. This is wasteful. Under hot, dry conditions, stomata close to conserve water, CO2 levels drop inside the leaf, and O2 levels rise relative to CO2. Photorespiration ramps up. C3 plants take the hardest hit from this. Some plants evolved workarounds. C4 plants spatially separate initial carbon fixation from the Calvin cycle. PEP carboxylase in mesophyll cells fixes CO2 into a four-carbon compound, which is then shuttled to bundle-sheath cells where CO2 is released at high concentration right around Rubisco. This effectively suppresses photorespiration. CAM plants do something similar but separate the steps temporally instead, opening stomata at night to fix CO2 and running the Calvin cycle during the day. Maize and sugarcane are classic C4 examples. Cacti and pineapples use CAM.
A common misconception is that more light always means more photosynthesis. That relationship plateaus. Once light saturation is reached, additional photons don't increase the rate because the Calvin cycle enzymes become the limiting factor. Further increasing light just creates excess energy that the plant must dissipate or risk damage. Similarly, raising CO2 concentration boosts photosynthesis only up to a point, and then other factors like temperature or nutrient availability take over as bottlenecks. Temperature matters a lot more than people expect. Enzyme kinetics in the Calvin cycle are temperature-sensitive. There is an optimal range, usually between 20 and 30 degrees Celsius for most C3 crops. Above that, enzymes denature and photorespiration increases. Below that, reaction rates slow dramatically. The Q10 effect means a ten-degree drop roughly halves the rate, and a ten-degree rise does the same until thermal damage sets in. If you are trying to measure or model photosynthesis in any real setting, you need to account for these interacting variables simultaneously. Isolating one factor in a controlled experiment is manageable. Replicating field conditions is not. Soil nutrient status, hydraulic conductivity, leaf age, and circadian rhythms all modulate the rate independently. A well-fed mature leaf under ideal conditions can run at gross photosynthetic rates exceeding 30 micromoles of CO2 per square meter per second. A stressed, nutrient-deprived leaf in full sun might manage less than five.
Get the Full Details
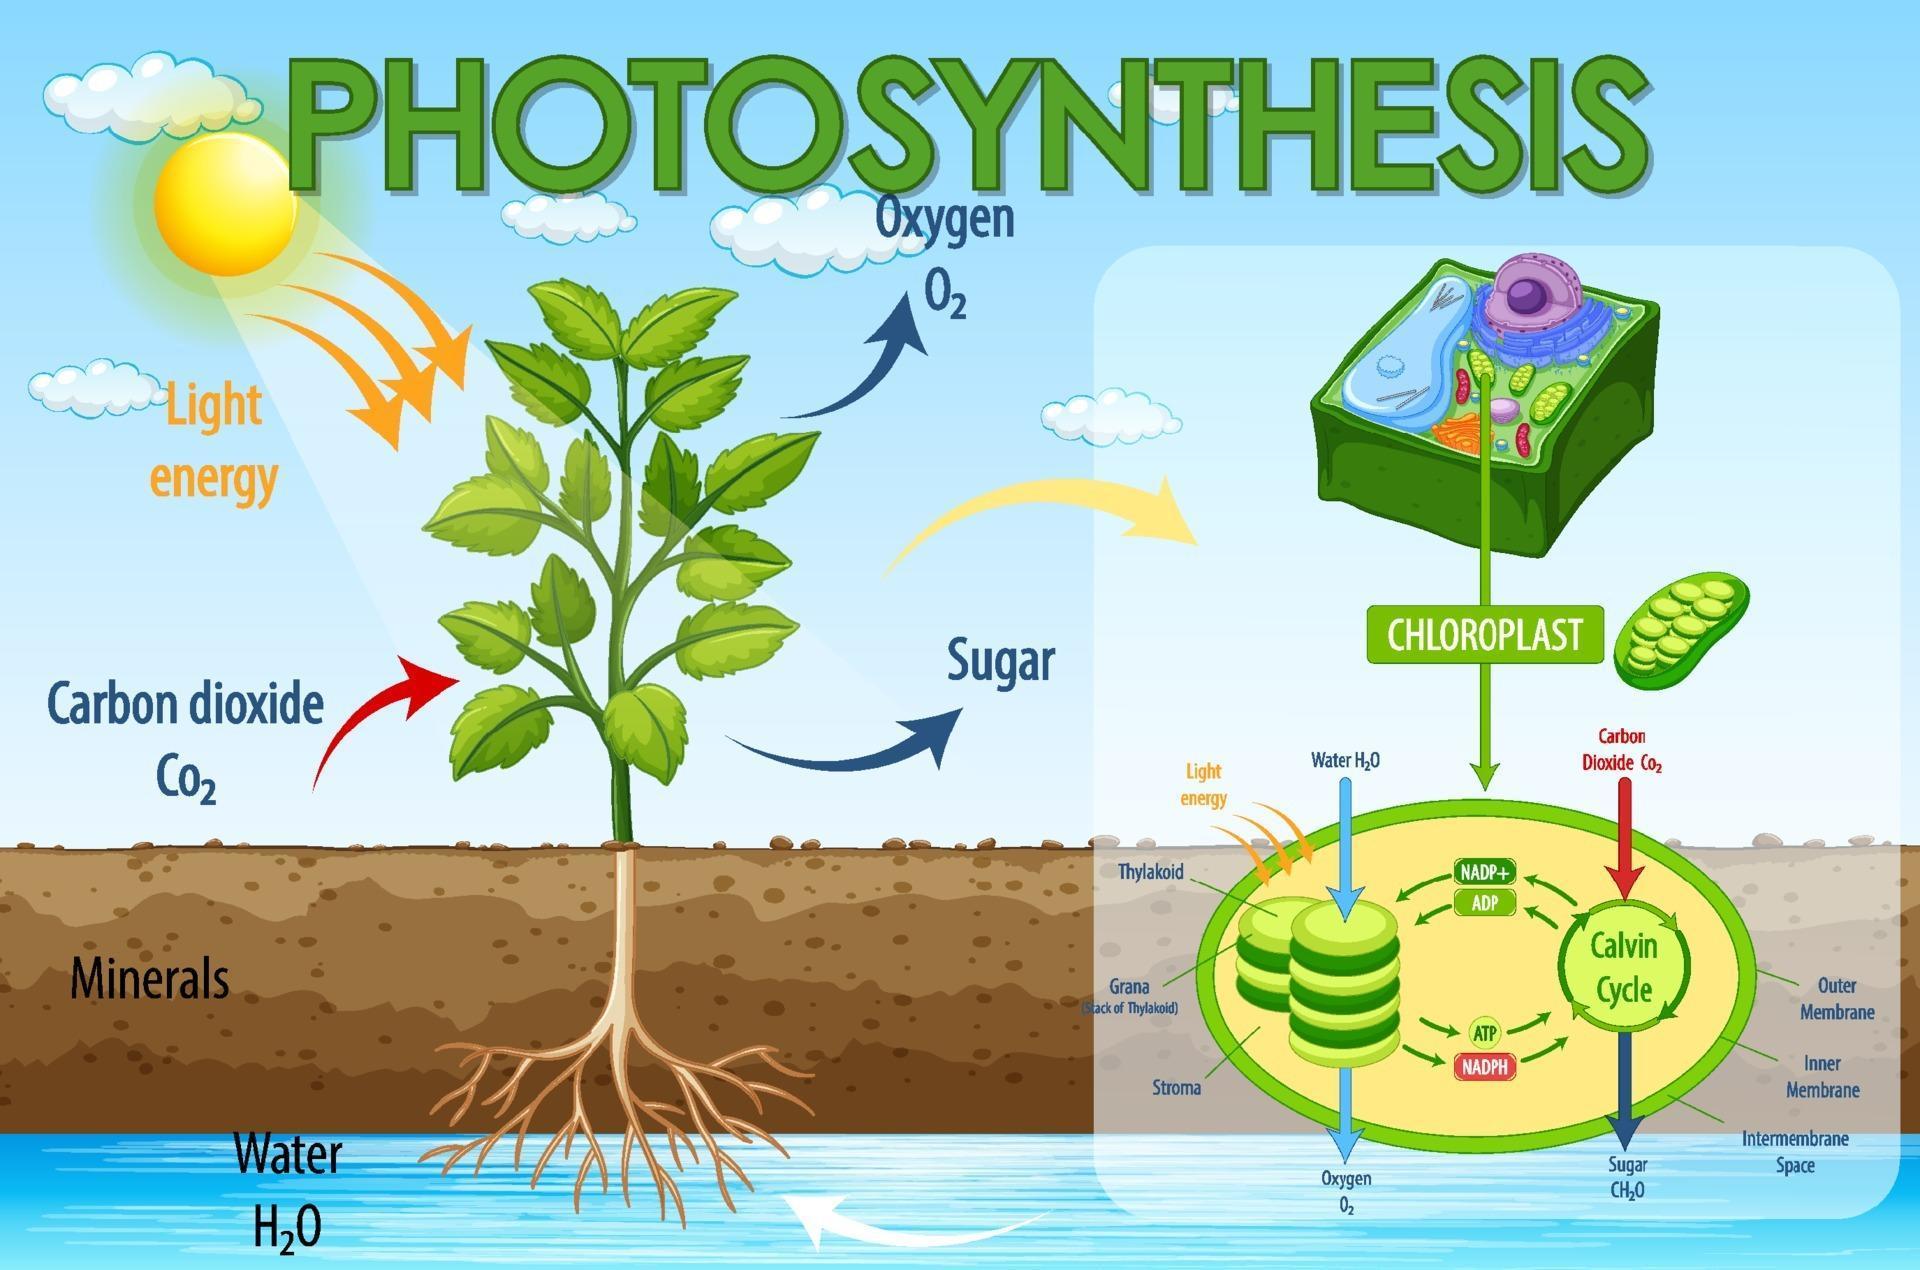
Understanding what photosynthesis is fundamentally changes how you approach anything involving plant productivity. Whether you are growing crops, designing a bioreactor with algal cultures, or just trying to keep a houseplant alive past the first winter, the constraints are always the same. Light, CO2, water, and temperature interact in ways that are rarely intuitive. The simplest mistake is assuming that maximizing one input linearly improves output. It does not.