The Difference Between Realized And Fundamental Niche Isn't As Simple As The Textbooks Make It Sound
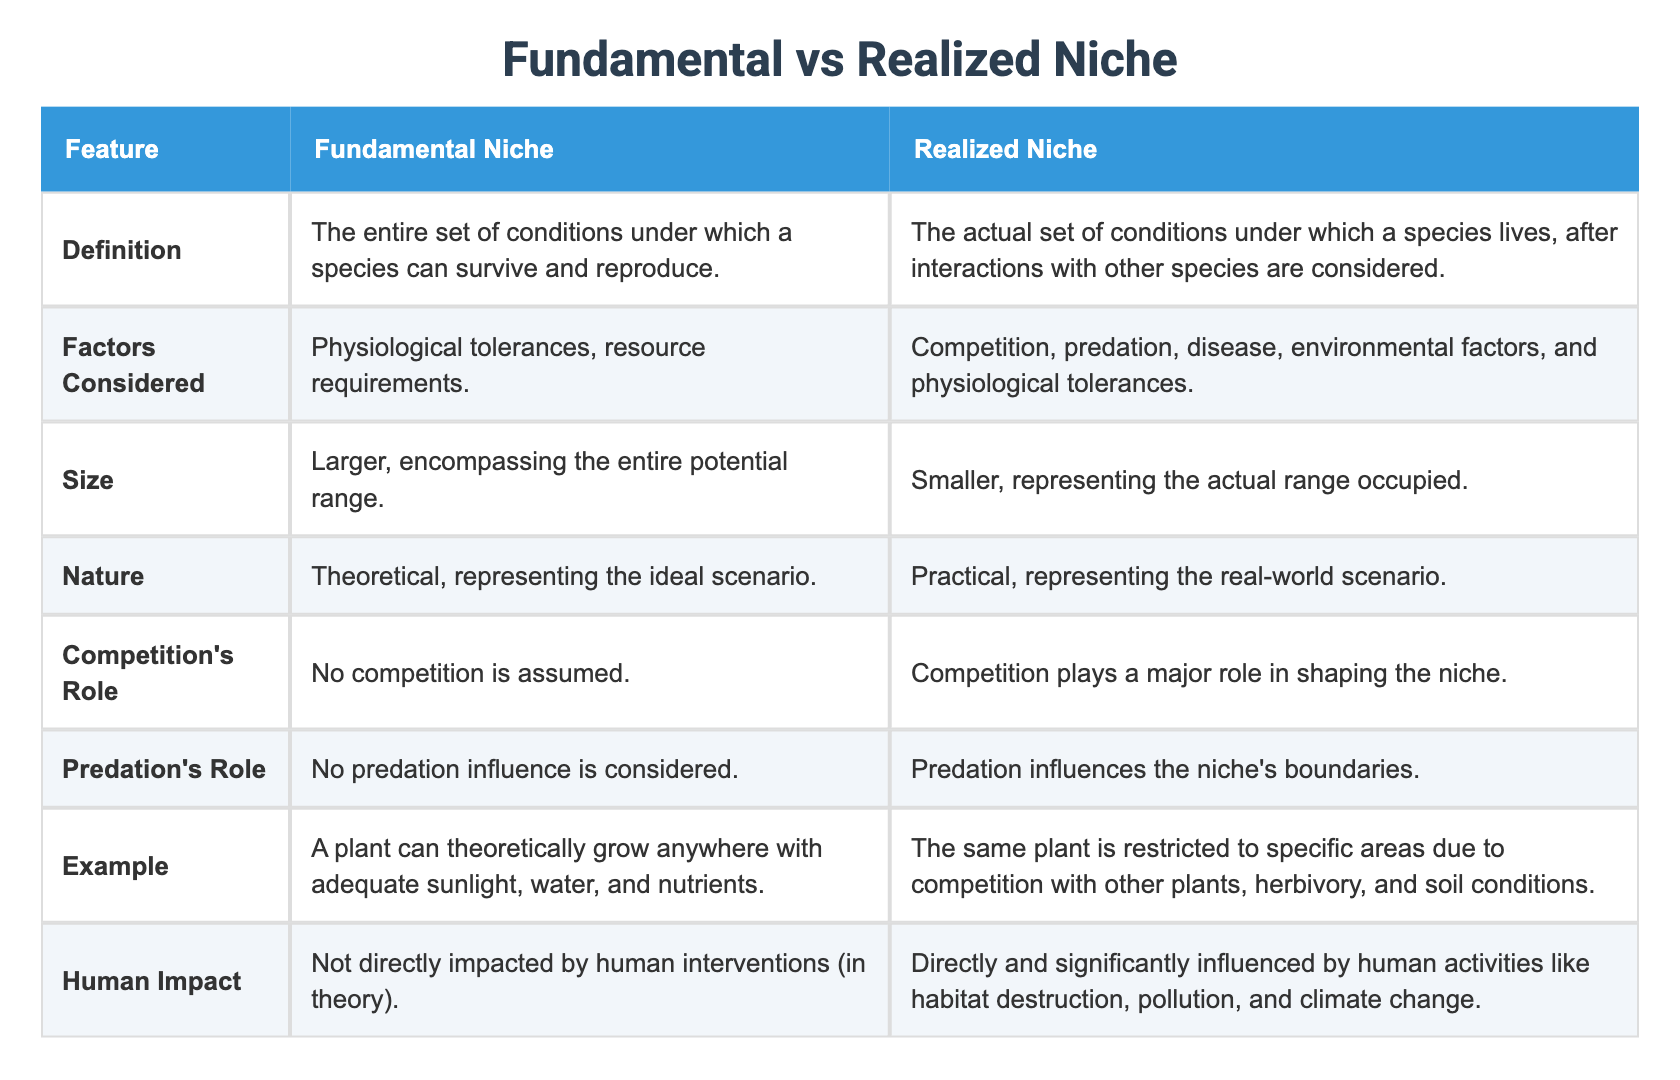
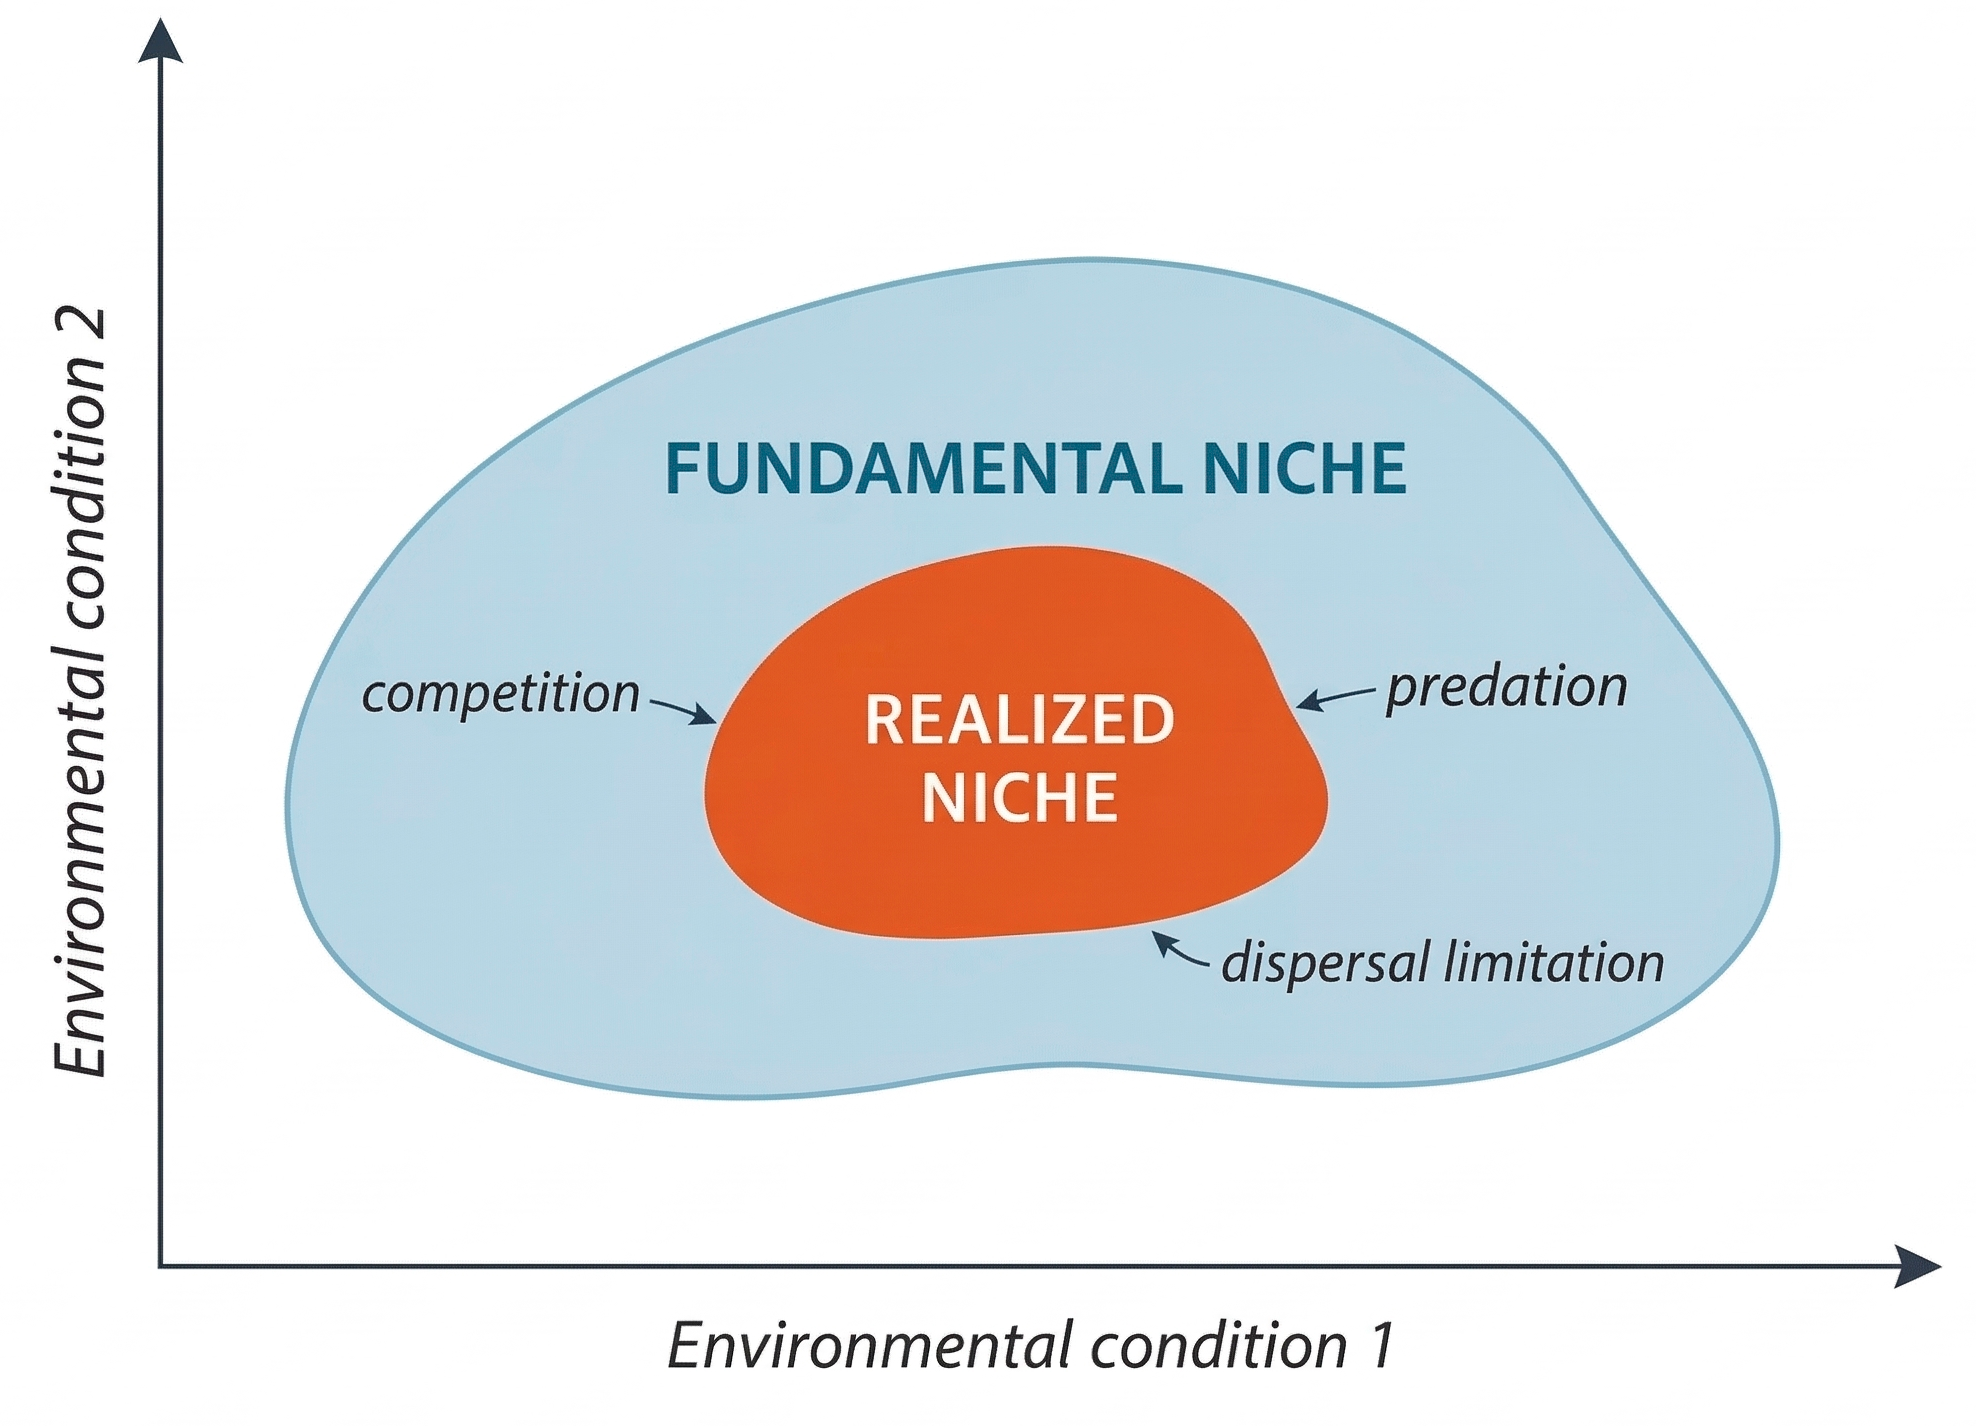
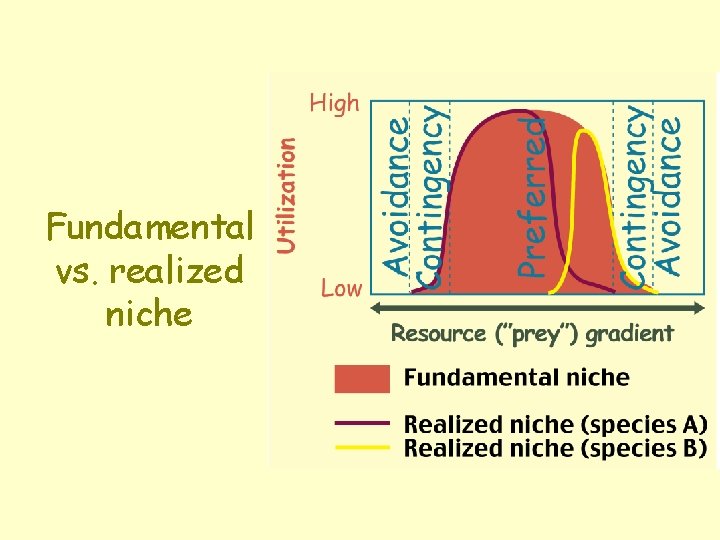
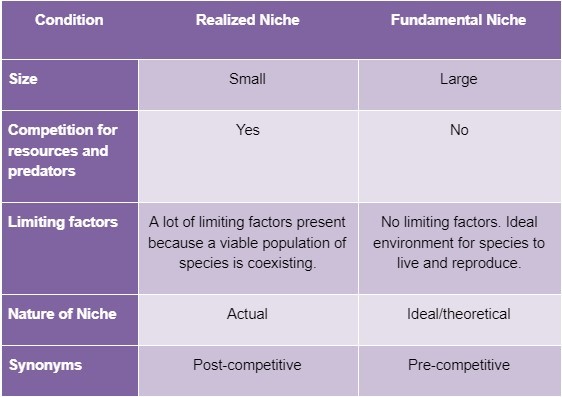
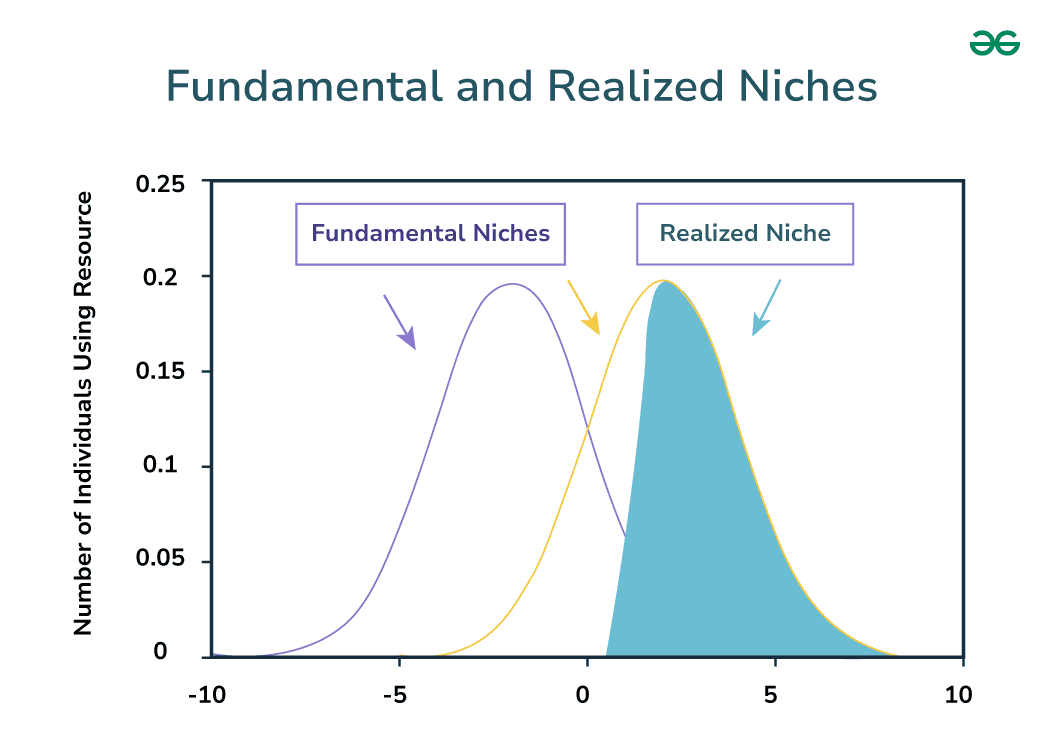
Most introductory ecology courses will hand you Hutchinson's definitions and move on. They'll tell you a fundamental niche is the full range of conditions under which a species can persist without competition, and a realized niche is what's left after competitors, predators, and other biotic interactions cut it down to size. That's correct. It's also mostly useless if you're actually trying to map niches in the field or model species distributions.
The problem starts when you try to operationalize these concepts. A fundamental niche isn't a fixed boundary you can just measure once and be done with. It shifts across generations when there's local adaptation, phenotypic plasticity, or genotype-by-environment interaction. If you're working with a widespread species like a perennial grass or a generalist pollinator, you'll find that populations at different elevations or latitudes have measurably different fundamental niches for the same trait — thermal tolerance, moisture requirements, flowering time. Treating the "fundamental niche" as a single envelope across a species' entire range will give you garbage outputs in any SDM or competition model.
Working With Realized Vs Fundamental Niche Data In Practice
When I've tried to pin down a fundamental niche experimentally, the quickest honest approach is a common garden or reciprocal transplant design across the environmental gradient you care about. You take individuals from multiple source populations, expose them across a controlled range of the focal variables, and measure performance metrics — survival, growth rate, reproductive output. The iso-performance contour that captures, say, the 50th percentile of fitness across all those treatments approximates the fundamental niche for that trait. It's not perfect. It doesn't capture evolutionary change over longer timescales, and it usually takes 6 to 18 months depending on the organism. But it's better than pulling a convex hull around occurrence records and calling it fundamental.
For the realized niche, you use occurrence or abundance data collected across environments where competitors are present. The standard approach here is a species distribution model — GLM, MaxEnt, random forest, whatever your team knows — using presence-absence or presence-only data with environmental layers. The difference between the two approaches shows you the narrowing effect of biotic interactions, assuming your environmental covariates are good enough to separate the abiotic filtering from the biotic part.
One thing people consistently get wrong is assuming the gap between fundamental and realized niche is always a contraction. It's not. Facilitation can expand the realized niche beyond the fundamental in harsh environments. I worked on a desert shrub project where the shrub's fundamental niche estimated from greenhouse experiments suggested it shouldn't survive below 300mm annual rainfall. But in the field, patches under the canopy of a dominant nurse plant persisted at 220mm. The realized niche was larger, not smaller, because the competitor was also a resource provider. Ignoring facilitation when comparing the two niches will make your models look broken and lead you to blame your environmental predictors instead of your ecological assumptions.
What Most Practitioners Miss About These Niches
The first counter-intuitive point is that the fundamental niche is often harder to define than the realized niche for a simple reason: biotic interactions, while complicated, leave measurable signatures in occurrence data. Abiotic limits require controlled experiments or mechanistic physiological measurements that are expensive and taxonomic-limited. For most taxa — insects, soil microbes, marine invertebrates — we don't have the physiological data to map fundamental niches well. We have distribution data. That means published "fundamental niche" maps in the literature are frequently just poorly filtered occurrence datasets masquerading as something more rigorous.
The second point is more practical. If you're building a model to predict how a species will respond to climate change or habitat fragmentation, what matters most isn't the difference between realized and fundamental. It's whether your environmental predictors are capturing the right axes of the niche. Temperature and precipitation are the usual defaults, but for a soil-dependent organism, pH, texture, and microbial community composition might be the actual limiting factors. I spent three months trying to reconcile modeled and observed ranges for a amphibian species until someone pointed out that our layer stack had no representation of soil drainage class. The model was predicting presence in suitable temperature bands that were actually impermeable clay. Adding a single soil layer fixed the mismatch.
There's also the issue of time lags. A realized niche map from current occurrence data may reflect historical conditions, not current equilibrium. Species trailing behind climate shifts — which is most of them — will show a realized niche that doesn't match the current environment. This is especially problematic when people use niche difference as a proxy for competitive ability in invasion biology. The invader might appear to occupy only a sliver of its fundamental niche because it hasn't reached equilibrium yet, not because competition is restricting it.
A Specific Edge Case I Ran Into
I was modeling a specialist wasp that parasitizes a single host beetle. The fundamental niche, derived from lab rearing across temperature and humidity gradients, suggested it could potentially establish in a broad swath of the coastal plain. The realized niche from trap data was fragmented into three disconnected patches. My initial hypothesis was competition or host limitation. Neither explained it. The breakdown came from realizing the lab experiments hadn't included the winter chill phase — these wasps require a prolonged cold period for diapause termination, and the coastal plain's winter temperatures had been warming past the threshold needed for proper development. The fundamental niche estimate was wrong because it was based on summer performance data only. Once I added winter minimum temperature as a constraint, the modeled fundamental niche collapsed to match the three observed patches almost exactly. The "gap" between niches wasn't biotic interaction at all. It was an incomplete experimental design.
This happens more often than you'd think. Most physiological niche studies focus on the conditions relevant to the active season. They skip over the overwintering, seed dormancy, or larval estivation phases where the real limits might sit. If you're doing this work, make sure your niche mapping covers the complete annual cycle of the organism, not just the part that's obvious.
When This Framework Fails
It fails completely when you're working with cryptic species complexes where morphological identification can't distinguish between multiple lineages that occupy genuinely different niches. I've seen this repeatedly in ground beetle and fungal groups. You run your niche models and get a realized niche that looks like a messy mixture of two or three distinct envelopes. No amount of statistical thinning or spatial filtering will clean that up. The fix is pre-screening with molecular data before you start niche work. It costs money and time upfront but saves you from spending six months chasing a pattern that doesn't exist.
It also breaks down for generalist species in highly disturbed landscapes where biotic interactions are so scrambled that the realized niche becomes more a reflection of disturbance regime than of competition or facilitation. In those cases, comparing realized to fundamental niche tells you something about disturbance intensity, not community structure. If your research question is about competition, pick a system where communities are relatively intact.
For practical purposes, if you need quick niche estimates and don't have physiological data, start with the realized niche from well-curated occurrence records using spatial filtering to reduce sampling bias. Use conservative environmental layers with resolution matching your study organism's dispersal scale. Then look for the gap between that and whatever fundamental niche data you can reasonably assemble. If the gap is large, investigate both biotic interaction and missing abiotic constraints before defaulting to the simpler explanation.
Gallery Realized Vs Fundamental Niche
Fundamental niche vs realized niche: why species do not occupy all the environments they could ...
Ecological niches Niches fundamental and realized Principle of
Realized niche Definition and Examples - Biology Online Dictionary
Ecological Niche Diagram 1729x1917
What Are Niche Examples at Jessie Nassar blog