What Actually Has To Be True For Natural Selection To Work
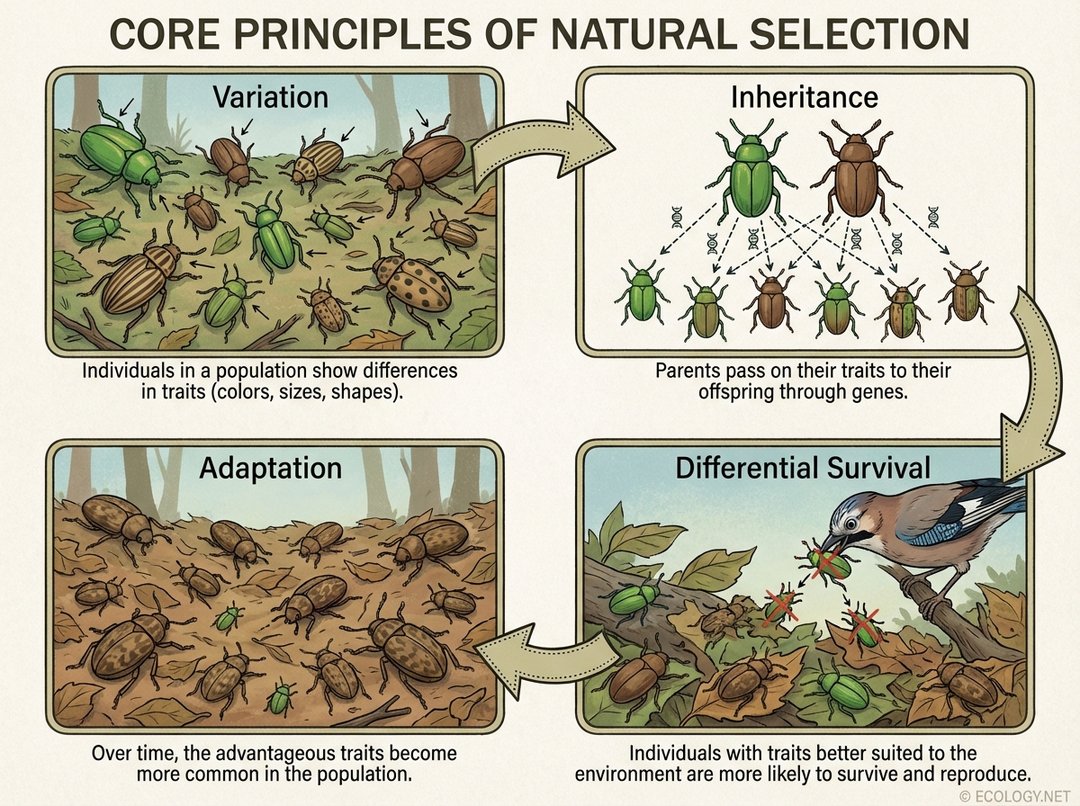
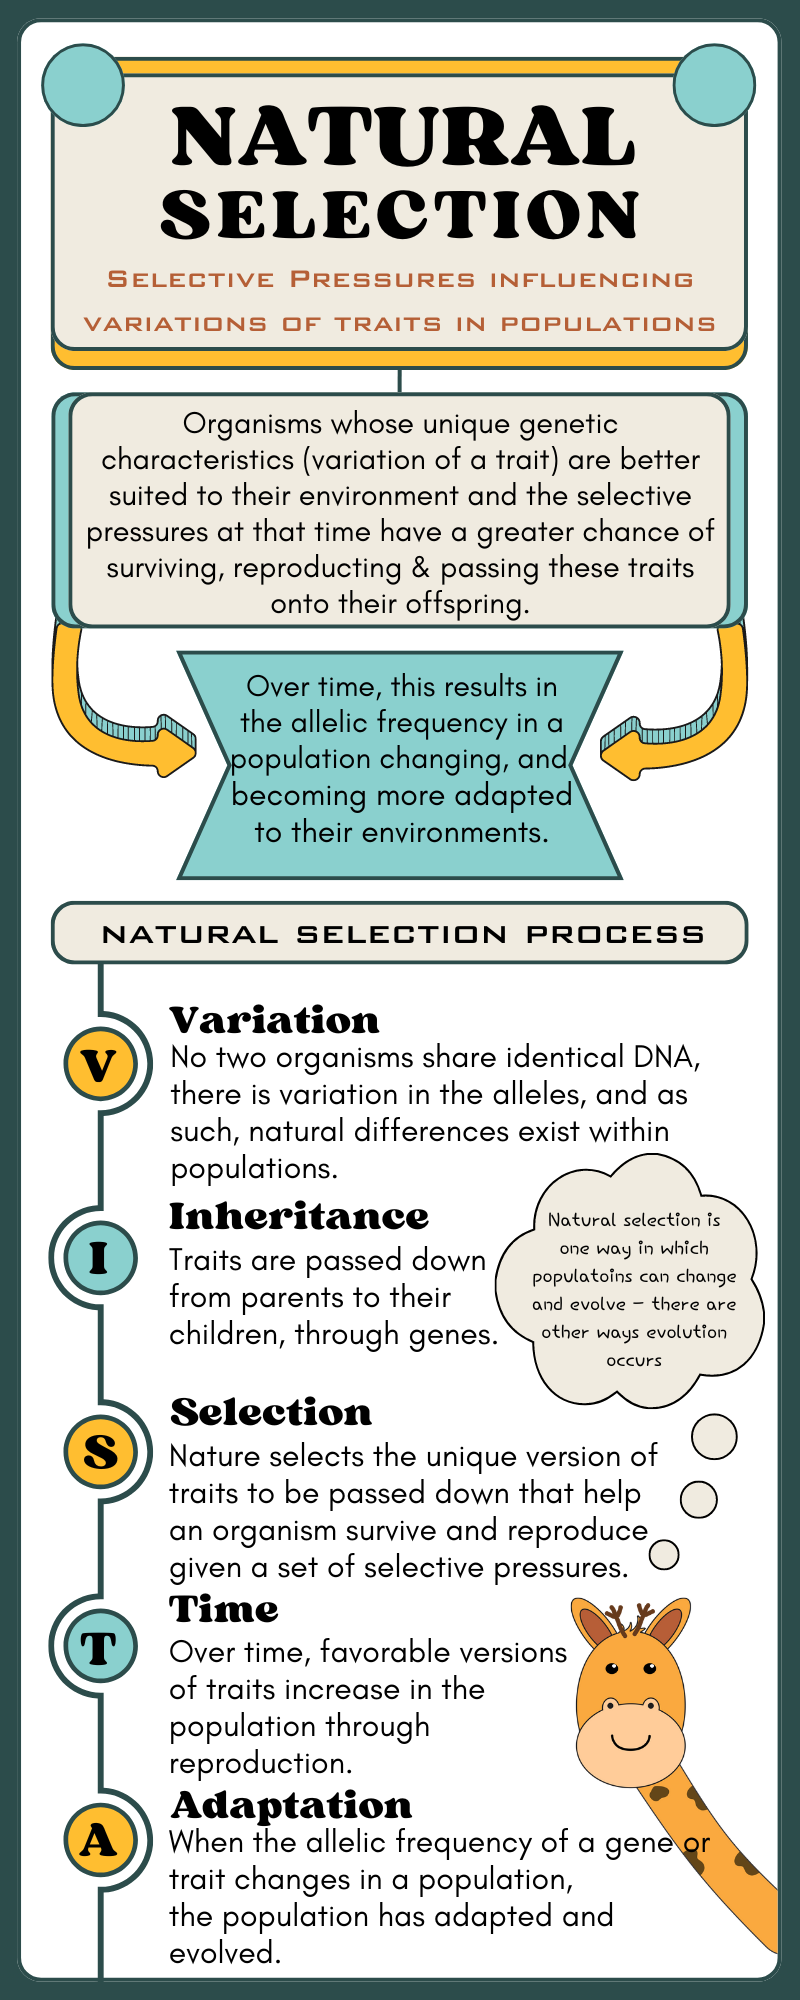
Everyone teaches the four requirements like they're a checklist. Variation. Heritability. Differential survival or reproduction. More offspring produced than can survive. You memorize that for an intro bio exam and move on. The reality is messier and more interesting. I spent years studying insect populations and watching selection play out in real time, which is how I learned that these requirements aren't just boxes to check. They interact with each other in ways that usually trip people up. Here is what actually matters when you are trying to understand or predict whether natural selection will happen in a given system.
Requirements For Natural Selection
Requirement one: there has to be heritable variation in the population. This sounds simple but people consistently miss the heritable part. I have seen students point to differences between individuals and assume natural selection is running. If the variation is purely environmental, it does not matter for evolution. A plant growing shorter because it is in shade is not a genetic difference. A plant growing shorter because it carries a certain allele is. You need the former for selection to do anything at all. I ran into this exact problem working on a population of beetles where body size varied massively across a gradient. My initial analysis showed strong size differentiation across microhabitats. I almost published it as evidence of directional selection until I realized the size differences were mostly plastic responses to temperature during development. The genetic component was basically zero. Three months of controlled common garden experiments later, I confirmed it and abandoned that particular hypothesis. Requirement two: that variation has to map to fitness differences. Not just survival. Reproduction matters more in most cases. A classic pitfall is assuming that a trait affecting survival automatically means selection. If the survivors are equally fecund, you have selection acting but no evolutionary response. I studied a moth population where parasitoid pressure strongly selected against darker morphs, yet the surviving light moths showed no difference in egg production. The population was undergoing selection without evolving. That distinction is critical for anyone modeling this stuff.
The fitness mapping is also usually nonlinear and context dependent. The allele that helps you in one environment hurts you in another. Spatial variation, temporal fluctuation, frequency dependence. I have watched a single locus maintain polymorphism through negative frequency dependent selection for over a decade in a lizard population. The homozygotes at both ends of the phenotypic range were selected against simply because they became too common. That is not a simple directional sweep. It is an equilibrium process that looks like stasis if you only sample occasionally. Requirement three: organisms have to overproduce relative to resources. Malthus understood this. Not every offspring survives. Not every gamete finds a partner. This is where the competitive element enters the model. Without excess production, every individual gets through, variation becomes irrelevant, and selection cannot sort anything. This requirement is easy to gloss over because it seems obvious. The hard part is measuring it in practice. In a long-lived tree species, annual seed output might be astronomically high, but recruitment is so sparse and spread over centuries that the selection differential is tiny per generation. You can satisfy the overproduction requirement and still get extremely slow evolutionary change because the generation time dilutes the selection pressure. I worked with a forestry team that misread this and predicted rapid adaptation to climate change based on seed output alone. They ignored the generation time problem. Wrong call. The trees were evolving, just on a timescale that made management relevance basically nonexistent for their lifespans.
Get the Full Details
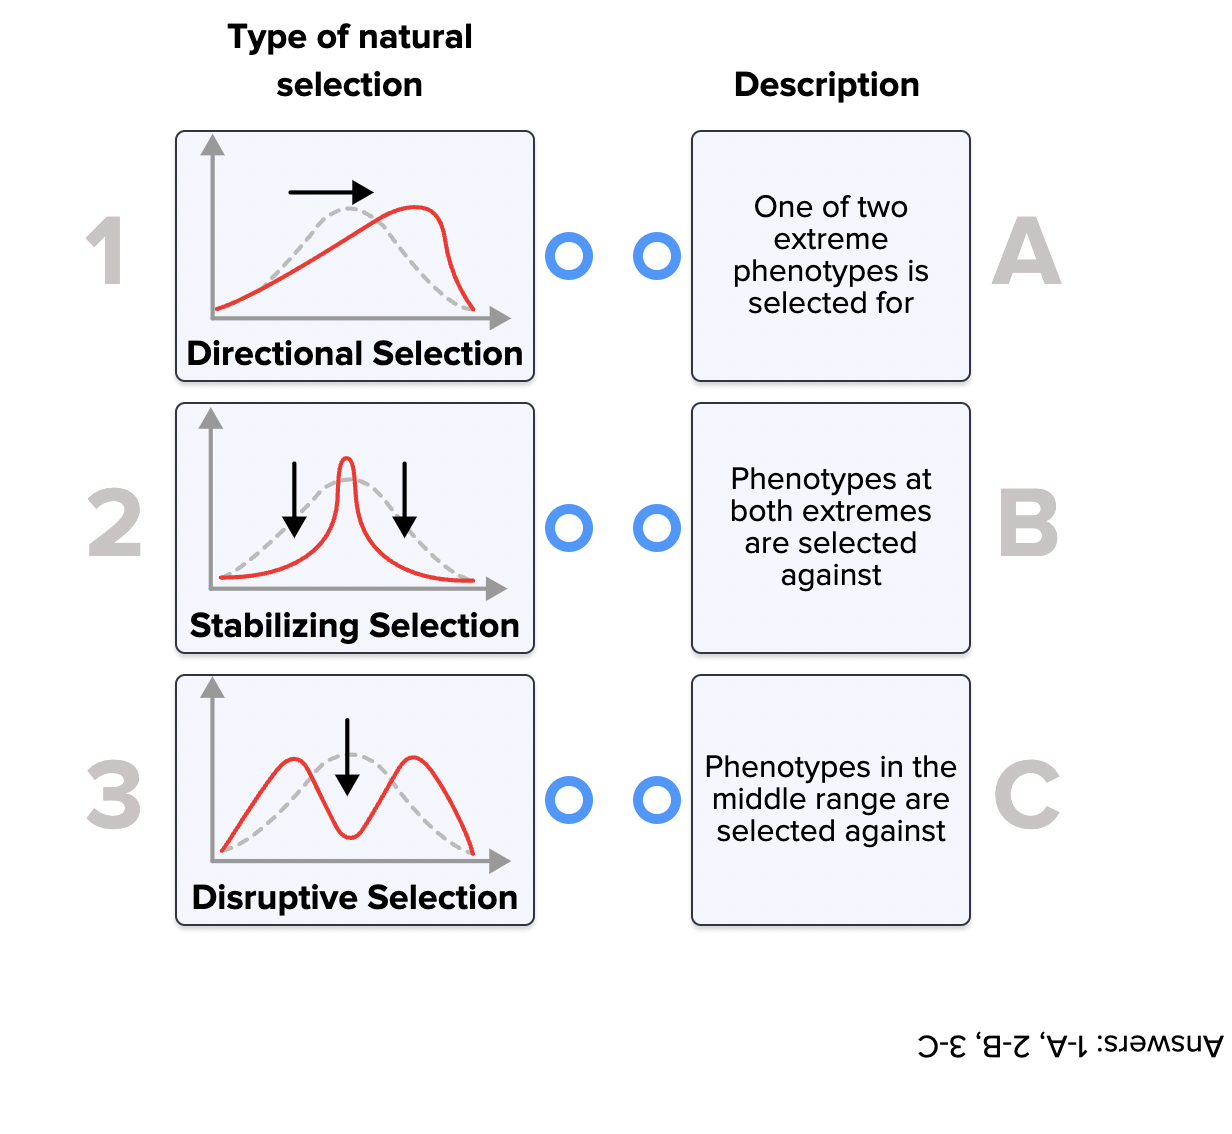
Requirement four: inheritance has to be reliable enough for selected traits to accumulate. This is the part most people conflate with the first requirement. Variation is one thing. Transmission is another. Recombination, mutation load, genetic drift, linkage disequilibrium. All of these can decouple the variation from the inheritance mechanism. I remember analyzing a population where the phenotypic variation looked substantial and the fitness differences were clear. The heritability estimates came back near zero because the relevant loci were locked in strong linkage disequilibrium with regions of low recombination. Selection was acting on the phenotype but could not shift the underlying allele frequencies fast enough. The population persisted in an evolved-looking but genetically static state for many generations. It took me a while to realize the selection was real and the inheritance was the bottleneck, not the other way around. There are additional nuances that rarely make it into textbooks. One is that natural selection does not require intelligence or intention. It is a statistical filter. Another is that selection on one trait can drag along correlated traits through pleiotropy or linkage, which means the observed changes are not always adaptive for the trait you are tracking. I have seen researchers attribute evolutionary change to selection on a focal trait when it was actually a correlated response, and they were pretty confident about it too.
The reverse is also true. Selection can act on a trait and produce no observable change if the genetic variance has been exhausted. I have encountered populations where the phenotypic distribution appeared static but the underlying genetic architecture was shifting quietly. That is called cryptic genetic variation and it shows up frequently under stress conditions. The variation was there all along, sitting in the genome, unrevealed until environmental conditions exposed it. If you are trying to test whether natural selection is operating in a system, the practical approach is to estimate the selection differential directly rather than infer it from phenotype distributions. Measure the trait in the population before selection and in the reproducing subset after selection. The difference is your selection differential. Then estimate heritability through breeding designs or genomic methods. Multiply the two and you get the predicted response. If the observed response matches the prediction, you have natural selection doing its thing. If it does not match, something is wrong with your assumptions about heritability, the fitness mapping, or the variance structure. I have also found that ignoring epistatic interactions leads to systematic errors in prediction. Most basic models treat additive genetic variance as sufficient. It often is. But in outcrossing populations with complex genotypes, epistasis can maintain hidden variance that additive models completely miss. When those conditions apply, the breeder's equation underestimates the evolutionary potential by a significant margin. I do not recommend building a full epistatic model unless you have the data for it, but you should at least be aware that the standard quantitative genetics framework has blind spots.
Natural selection is not a force that pushes populations toward perfection. It is a filtering process that removes combinations that fail to reproduce relative to others in the same environment. The environment changes, the filter changes, and the direction changes with it. That is why populations are never optimally adapted, only sufficiently adapted to persist in their current conditions. The requirements are necessary but they do not guarantee a predictable outcome.