Getting Your Head Around the Two Types of Endoplasmic Reticulum
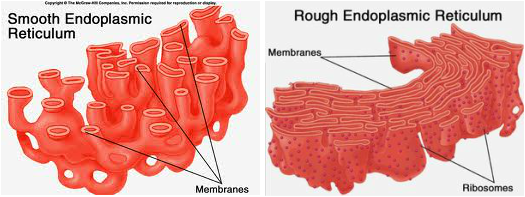
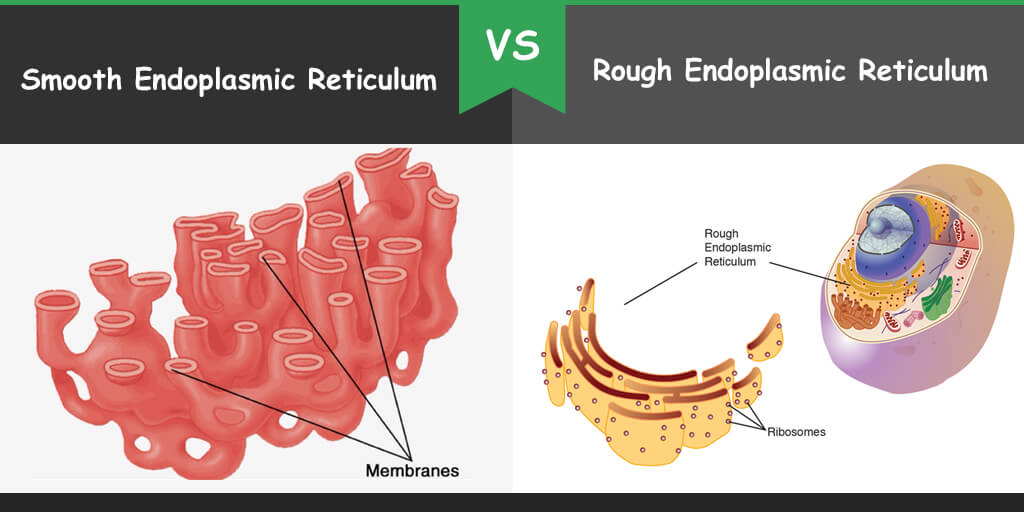
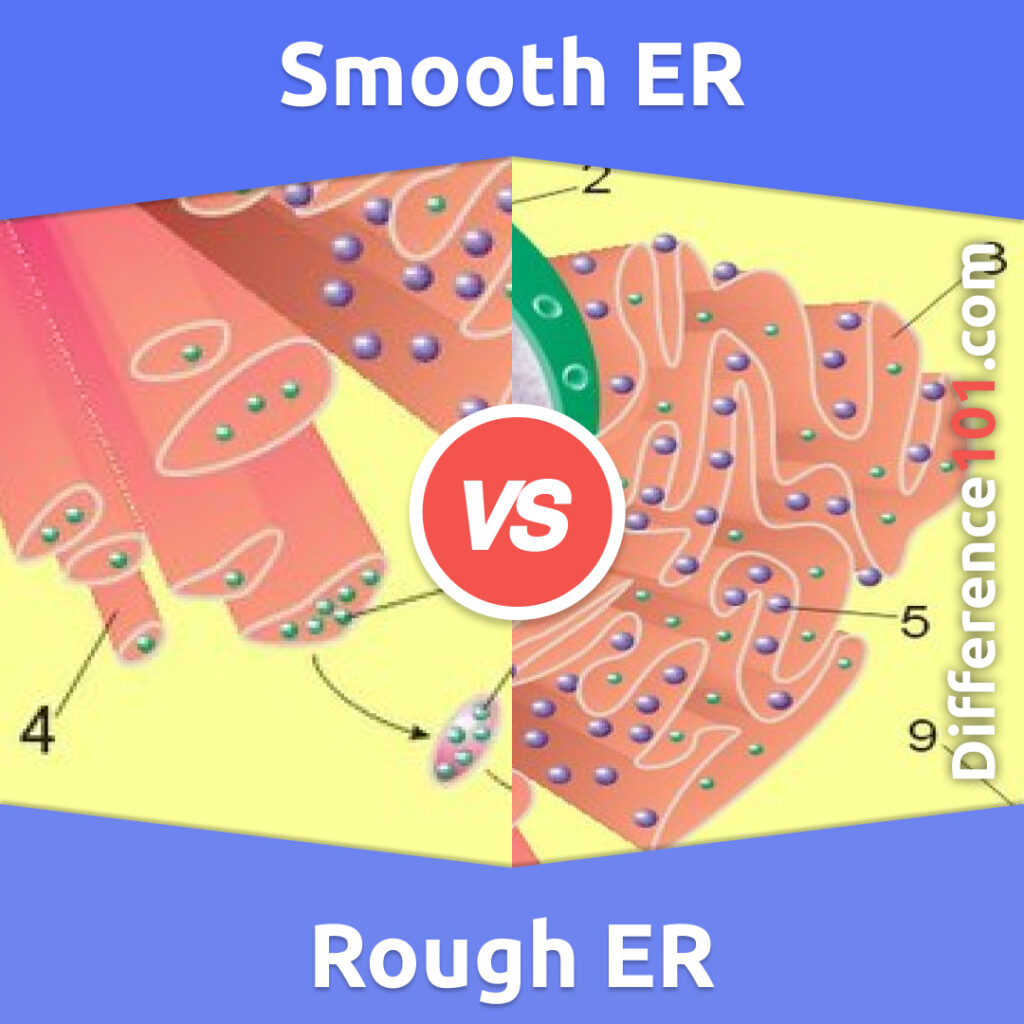
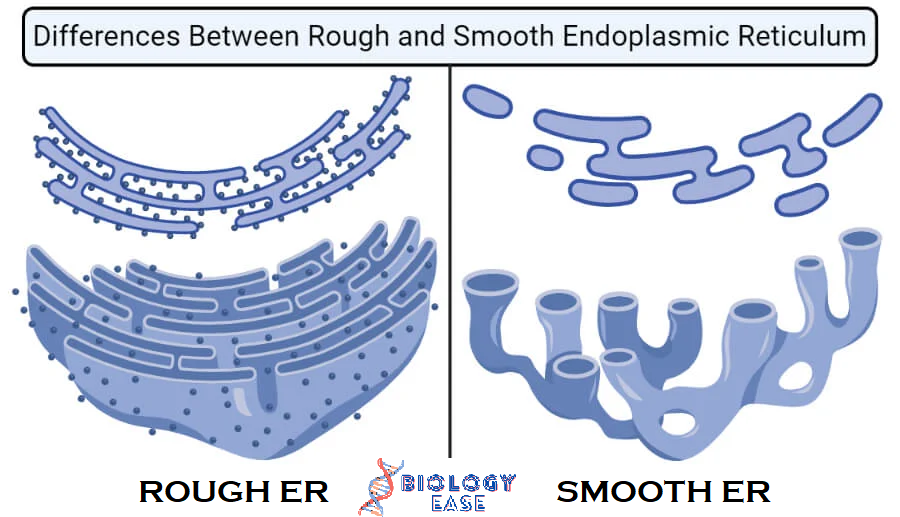
You look at a cell under an electron microscope and you see this tangled network of membranes. Some parts look bumpy. Some parts look clean and tubular. That bumpiness is ribosomes stuck to the outside, and that's the single most important visual difference between rough and smooth ER. Everything else about them follows from that basic structural fact. I spent years working with cell fractionation protocols, and one thing that always trips people up is assuming these two types exist as separate physical compartments in every cell. They don't. They're continuous with each other. The rough ER transitions directly into smooth ER depending on what that region of the membrane is doing. A single cell can have patches of both side by side, and which one dominates depends entirely on the cell's current function. Hepatocytes, for instance, have massive amounts of smooth ER because they're processing drugs and toxins. Pancreatic acinar cells are packed with rough ER because they're churning out enzymes for secretion.
Rough Er Vs Smooth Er
The rough ER's job is protein synthesis and initial modification. Ribosomes dock onto translocon channels in the membrane and feed nascent polypeptide chains into the lumen. Inside that lumen, you've got chaperones like BiP folding proteins, glycosylation enzymes adding N-linked sugars, and disulfide bond formases helping structure stabilize. Proteins destined for the secretory pathway — membrane proteins, lysosomal enzymes, extracellular matrix components, hormones — all go through here first. If something goes wrong with folding, the ER retention machinery catches it and targets it for degradation via ERAD, which is ER-associated degradation, not to be confused with proteasomal degradation that happens in the cytoplasm. The smooth ER handles lipid synthesis, calcium storage, and detoxification. No ribosomes means no protein manufacturing. Instead you've got enzymes embedded in the membrane that synthesize phospholipids and cholesterol, which then get ferried to other membranes via lipid transfer proteins or vesicular transport. In muscle cells, the smooth ER is specialized into the sarcoplasmic reticulum, and it's ridiculously efficient at pumping calcium back up after contraction. Take-away that function and you get sustained tetanic contraction, which is basically how certain venoms and toxins work. Here's a detail most textbooks skip: the smooth ER isn't just a passive storage tank for calcium. It actively participates in signal transduction. When IP3 receptors on the smooth ER membrane open in response to signaling cascades, calcium floods into the cytoplasm and triggers everything from neurotransmitter release to gene expression changes. The concentration gradient across the ER membrane is about 10,000-to-1. That's not a small difference. It's a loaded spring.
One practical problem I ran into repeatedly when isolating ER fractions: the rough and smooth ER don't separate cleanly by standard differential centrifugation. They're interconnected, and rough ER tends to fragment into smaller vesicles during homogenization, while smooth ER forms larger tubular networks. I ended up using a combination of Sucrose density gradients and selective detergents that preferentially solubilize one type over the other. The key was keeping the samples cold and working fast. Once the membranes start breaking down, you lose the structural distinction entirely and your downstream assays become meaningless. If you're trying to study just one type functionally, the workaround I found reliable was using cell lines where one pathway is genetically upregulated. For rough ER studies, induce heavy secretory protein production with tunicamycin stress or overexpress a secretory protein tagged with GFP. For smooth ER, use conditions that demand lipid synthesis — low-density lipoprotein stimulation in hepatoma cells, for example. That shifts the balance visibly under microscopy without requiring microdissection, which basically isn't practical at the subcellular level. The counter-intuitive thing about rough ER is that it's not just about making more protein. Quality control is the real bottleneck. A cell can produce proteins fast, but if the folding capacity is exceeded, the unfolded protein response kicks in and actually shuts down translation globally. I've seen cultures where protein output dropped by half simply because the ER was overwhelmed. Adding more ribosomes doesn't solve that. You need to expand the chaperone capacity or reduce the folding burden.
Get the Full Details
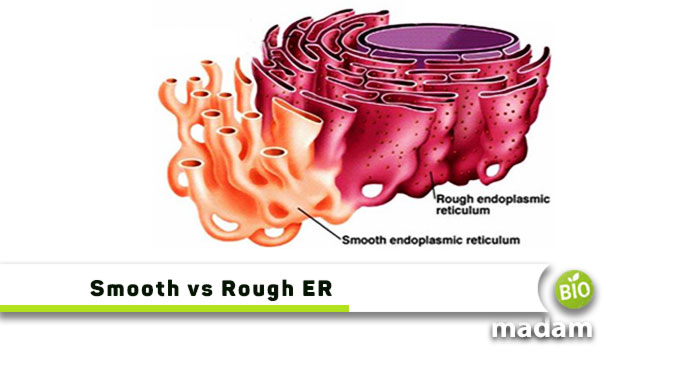
For smooth ER, the common misunderstanding is that it's just the "other one." It's actively doing things the rough ER literally cannot do. Drug-metabolizing enzymes like the cytochrome P450 family are embedded exclusively in smooth ER membranes. These handle oxidation, reduction, and conjugation reactions that make hydrophobic compounds water-soluble for excretion. Chronic exposure to certain drugs literally increases smooth ER membrane volume in liver cells. That's enzyme induction, and it's why dosage adjustments are sometimes necessary after prolonged medication. Both types share the same basic membrane architecture — a phospholipid bilayer with integral and peripheral proteins. The lumen is topologically equivalent to the extracellular space, which matters for things like glycosylation. Anything inside the ER lumen is technically outside the cell from a membrane topology standpoint. This is also why the ER is the first checkpoint for the secretory pathway. The biggest pitfall I see people make is treating rough and smooth ER as fixed categories rather than functional states of a dynamic membrane system. They're not separate organelles in the way mitochondria are. They're regions of the same reticulum adopting different shapes and functions based on cellular demand. The membrane curvature, protein composition, and lipid content all shift continuously between rough and smooth domains.