Understanding the Glycolytic Pathway from the Bench Up
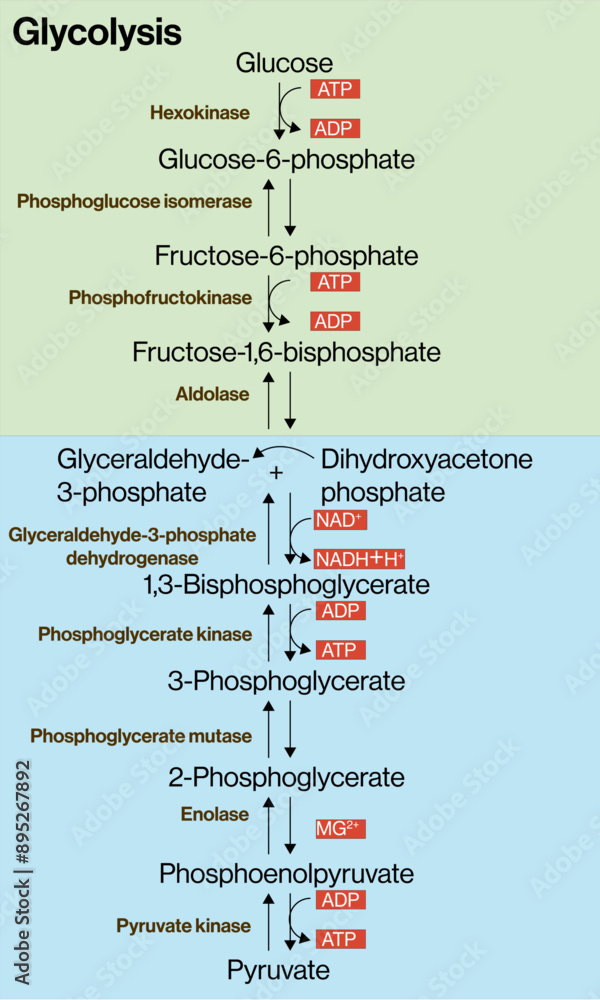
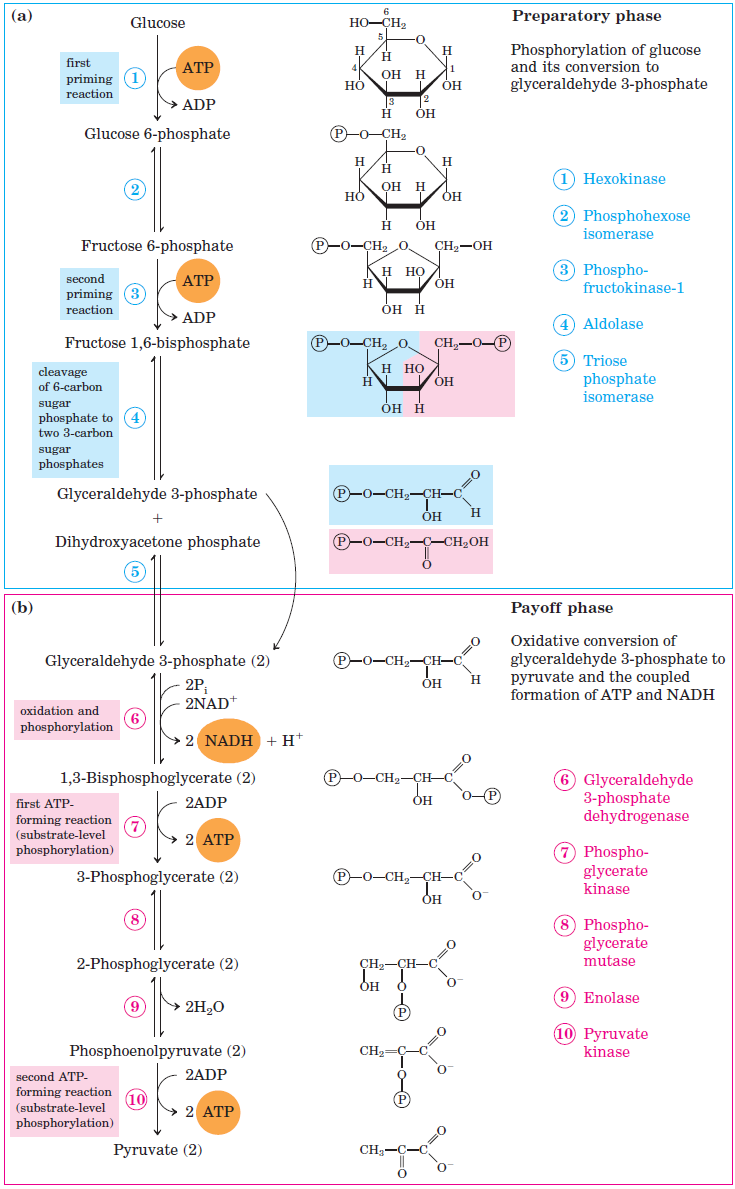
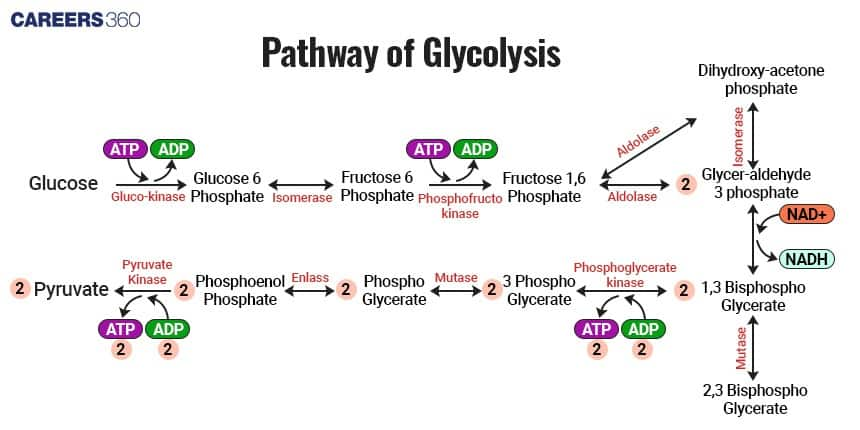
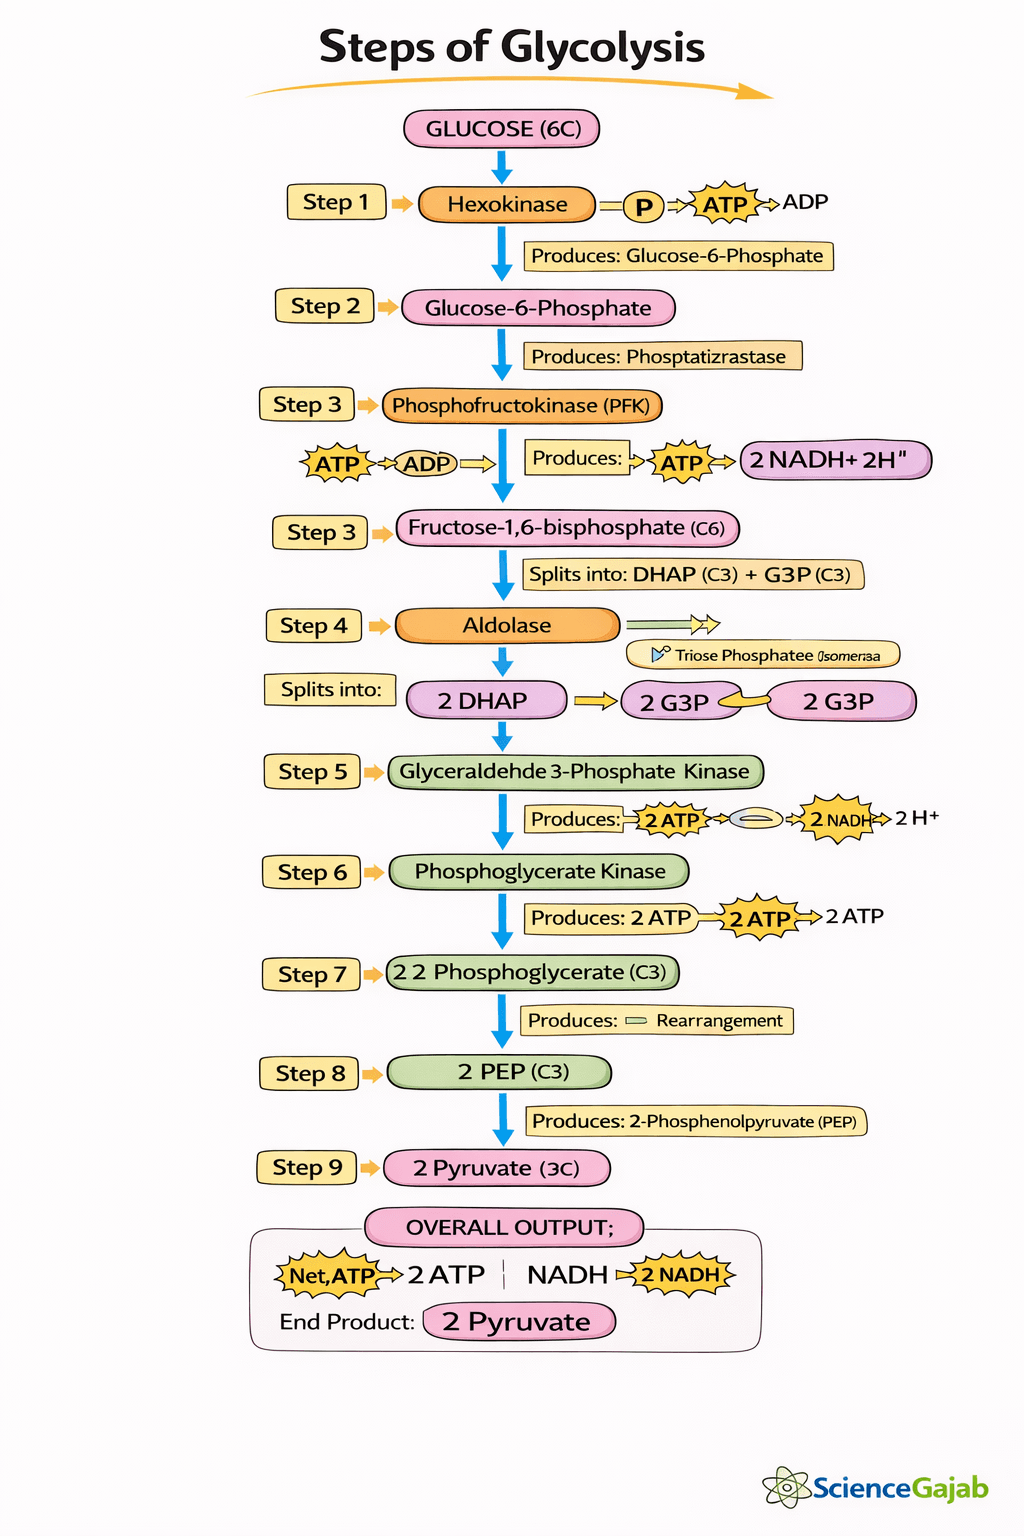
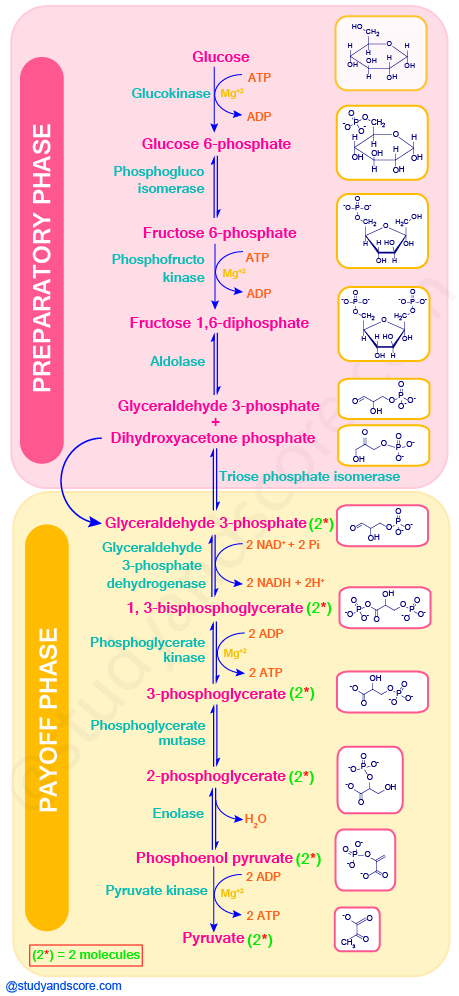
Glycolysis is ten enzyme-catalyzed reactions that convert one molecule of glucose into two molecules of pyruvate, producing a net gain of two ATP and two NADH in the process. It takes place entirely in the cytoplasm. Most textbooks lay it out as two phases—an investment phase consuming two ATP and a payoff phase generating four ATP—but that framing misses what actually matters when you are working with cells in a real experiment. The first three steps form the preparatory segment. Glucose enters the cell and gets phosphorylated by hexokinase at the expense of one ATP, trapping it inside because glucose-6-phosphate cannot cross the membrane. That phosphorylation is effectively irreversible under physiological conditions. Phosphoglucose isomerase then converts glucose-6-phosphate into fructose-6-phosphate, a simple aldose-to-ketose rearrangement that most people breeze past but is worth paying attention to because it sets up the next step. Phosphofructokinase-1, or PFK-1, uses a second ATP to phosphorylate fructose-6-phosphate into fructose-1,6-bisphosphate. This is the main regulatory checkpoint in the entire pathway. PFK-1 responds to energy charge, citrate levels, and pH. When ATP is high, PFK-1 slows down. When AMP is high, it speeds up. Citrate from the mitochondria also inhibits it, which is how the cell coordinates glycolysis with the citric acid cycle. Aldolase splits fructose-1,6-bisphosphate into two three-carbon molecules: dihydroxyacetone phosphate and glyceraldehyde-3-phosphate. Triose phosphate isomerase converts the DHAP into a second molecule of G3P so both carbons can continue through the payoff phase. You start with one glucose and end up with two molecules of G3P, which is why every reaction after this point happens twice per glucose.
Step By Step Of Glycolysis: What Actually Happens in the Payoff Phase
Glyceraldehyde-3-phosphate dehydrogenase catalyzes the oxidation and phosphorylation of G3P. Inorganic phosphate is incorporated and NAD+ is reduced to NADH. This is the only step in glycolysis that generates NADH directly. If the cell cannot regenerate NAD+, this reaction stops and the whole pathway grinds to a halt. That is not theoretical. I ran an experiment a few years ago where I deliberately limited oxygen in a yeast culture to observe the shift from aerobic respiration to fermentation, and within about twenty minutes the intracellular NAD+ pool was depleted enough that lactate dehydrogenase kicked in to recycle it. The moment I restored aeration, the NADH oxidized back through the electron transport chain and glycolysis accelerated again. Tracking this in real time with a spectrophotometer reading absorbance at 340 nanometers gave me a clean kinetic curve, but it also made clear that NAD+ availability is the hidden bottleneck nobody talks about in introductory courses. Phosphoglycerate kinase transfers a phosphate from 1,3-bisphosphoglycerate to ADP, making ATP and 3-phosphoglycerate. This is substrate-level phosphorylation. Next, phosphoglycerate mutase moves the remaining phosphate from carbon 3 to carbon 2, producing 2-phosphoglycerate. Enolase then dehydrates that intermediate to form phosphoenolpyruvate, a high-energy compound. Finally, pyruvate kinase converts PEP to pyruvate while generating another ATP per molecule. Two pyruvate molecules result from one glucose, and the net yield is two ATP plus two NADH. The pyruvate kinase step is another irreversible reaction and a secondary control point. It is activated by fructose-1,6-bisphosphate, which is a feed-forward mechanism linking the early commitment step to the final ATP-generating step. It is inhibited by ATP and alanine. When alanine is high, the cell has plenty of biosynthetic precursors and there is no need to keep pushing glucose through the pathway.
Here is something most students miss. The textbook number of two net ATP assumes ideal conditions, but the actual yield depends on the shuttle system moving NADH from the cytoplasm into the mitochondria. The malate-aspartate shuttle preserves the reducing power and yields about 2.5 ATP per NADH, while the glycerol-3-phosphate shuttle loses some energy and yields closer to 1.5 ATP per NADH. So depending on tissue type, your total from glycolysis alone could be three or four ATP equivalents when you count the NADH, not just the substrate-level two. Another practical consideration is the effect of pH on phosphofructokinase. In working muscle during intense exercise, accumulating protons inhibit PFK-1 directly. This is why glycogenolysis can actually compete with glycolysis for intermediates when the cell is acidic. I have seen cases in exercise physiology labs where researchers assumed lactate buildup was purely a product of high flux, but the data showed the opposite direction at times: the acidosis itself was throttling glycolytic flux and forcing a metabolic shift. The takeaway is that glycolysis is not a rigid assembly line. It is a regulated network with multiple feedback loops responding to energy status, substrate availability, and cellular conditions. If you are trying to manipulate glycolysis experimentally, the most reliable targets are hexokinase, phosphofructokinase-1, and pyruvate kinase. Inhibiting any of these with compounds like iodoacetate for GAPDH or fluoroacetate upstream will shut down the pathway predictably, but the downstream effects cascade in ways that are easy to misinterpret. Always measure both ATP and NADH levels simultaneously when testing inhibitors, because changes in one do not always predict changes in the other.
Get the Full Details