What Actually Happens When a Cell Divides
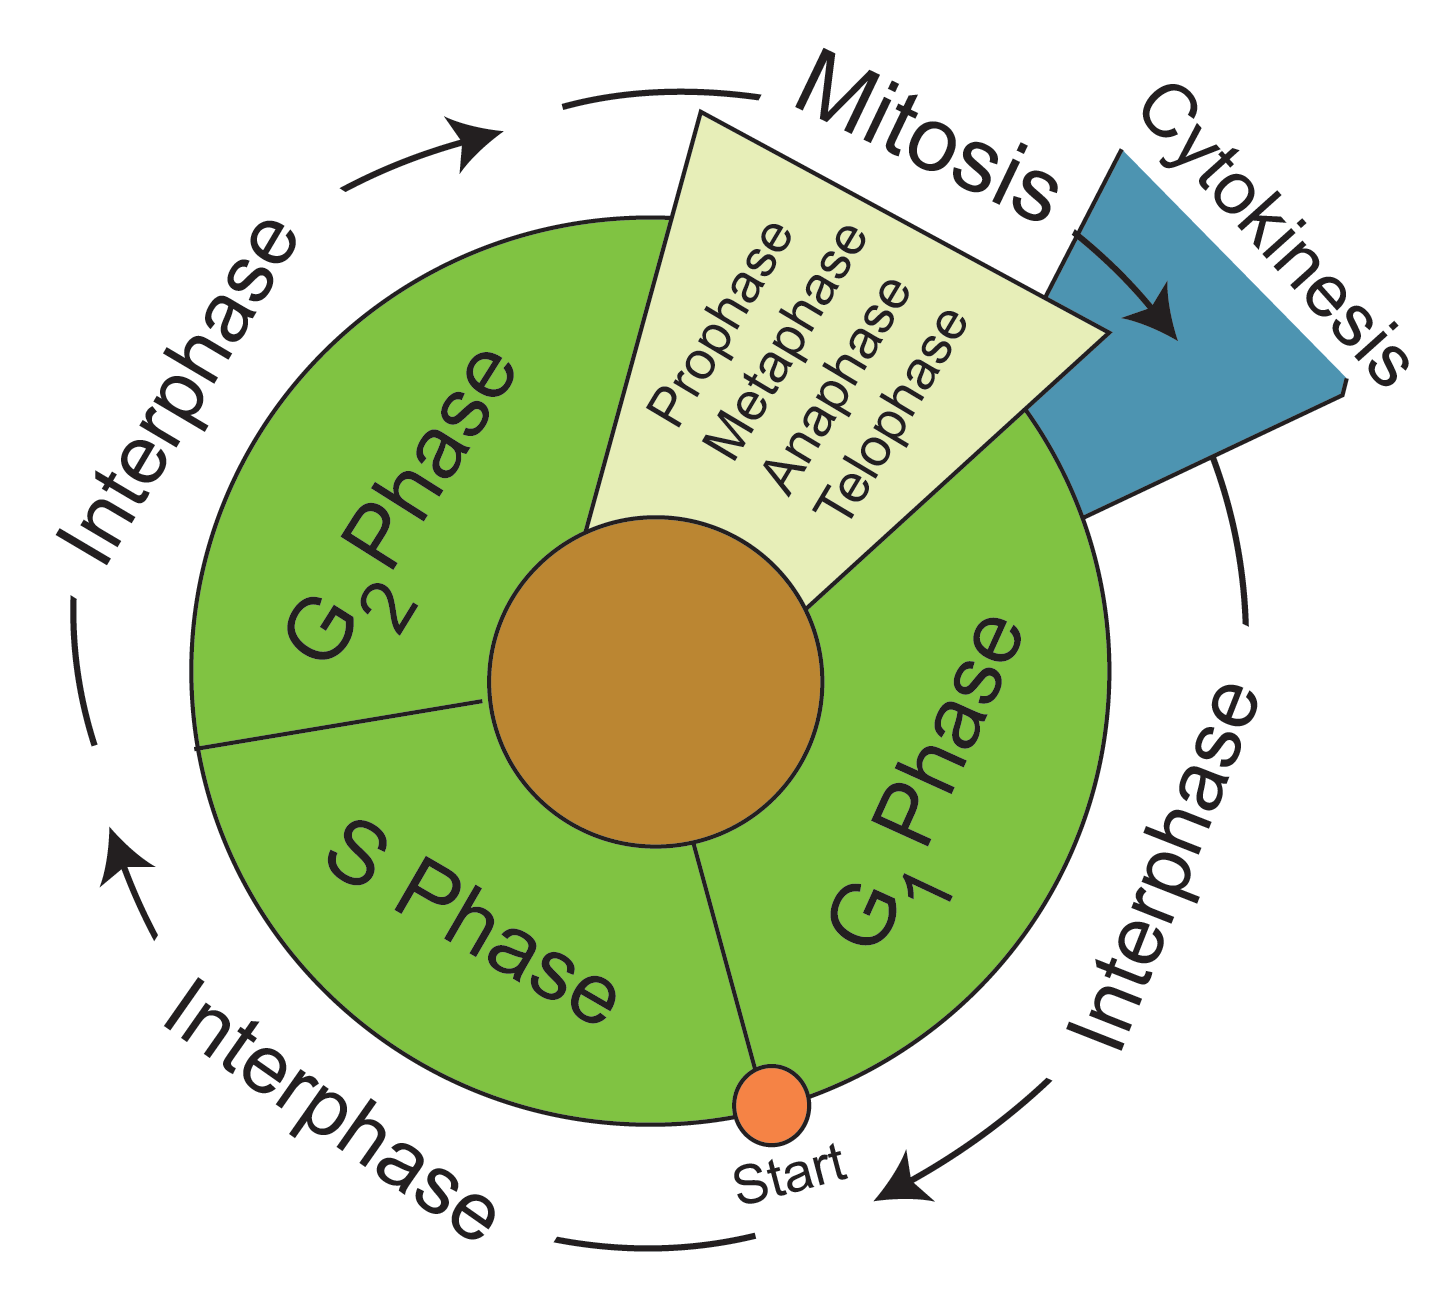
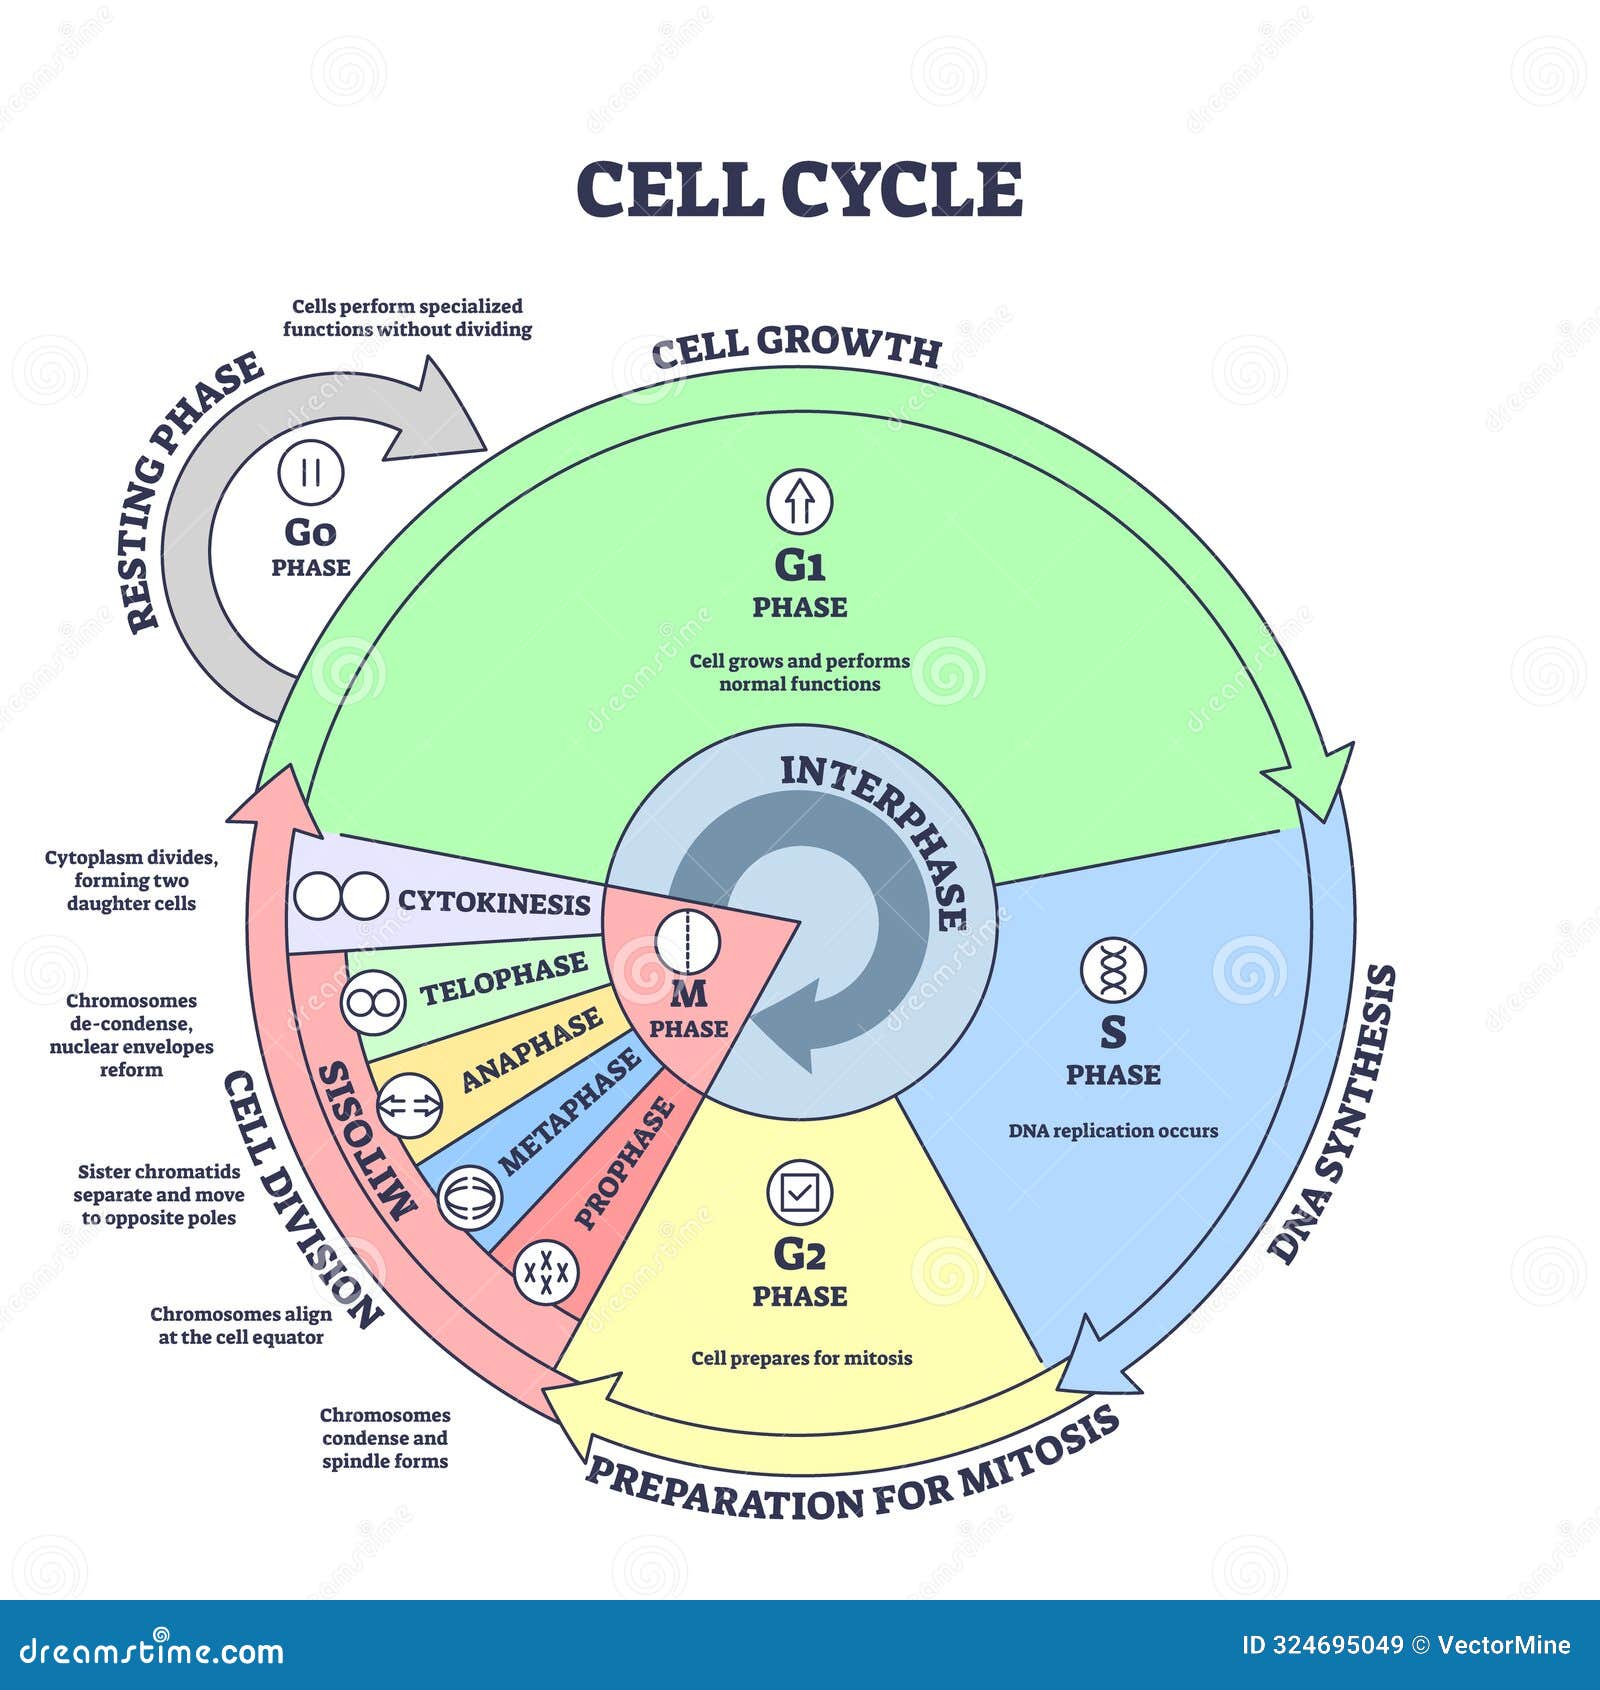
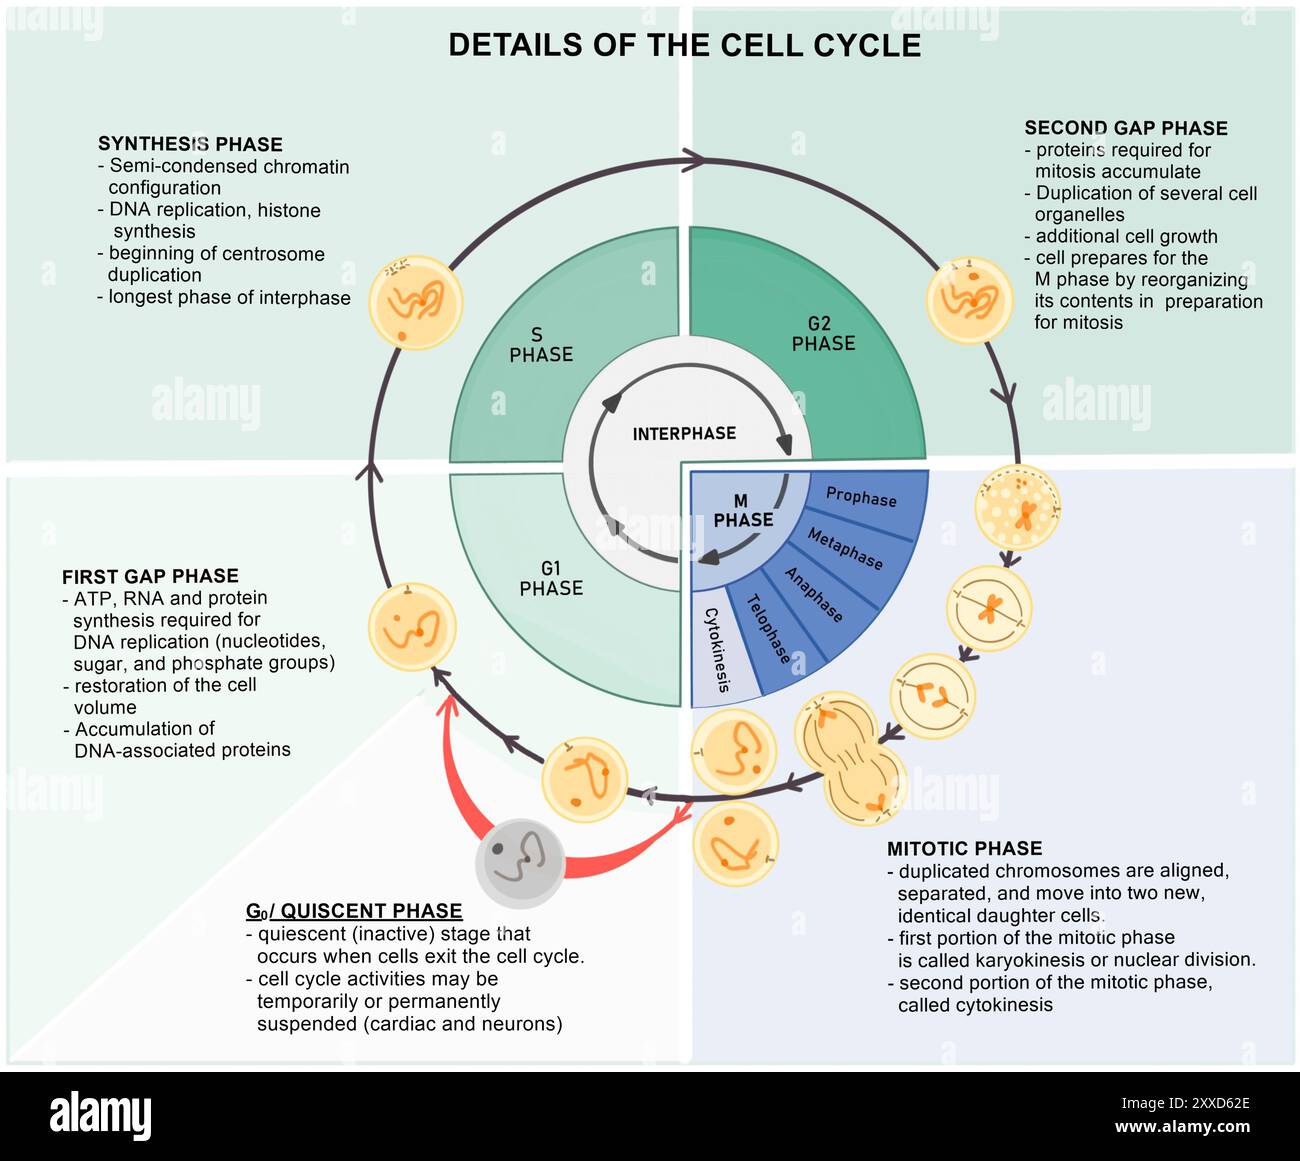
The cell cycle is just a repeating series of events that turns one cell into two. It is not complicated if you stop trying to memorize it as a list and instead understand why each step exists. I spent years working with cell culture, and the people who actually get it are the ones who think about checkpoints and failure modes, not the ones who recite phases back to you. There are four main phases. G1, S, G2, and M. Between divisions there is also G0, which is basically the cell saying it is done and going to sit there until something tells it otherwise. Here is how they actually play out in practice. G1 is the first gap phase. The cell grows, makes proteins, and checks whether conditions are even worth dividing in. This is where most of the regulation happens. If nutrients are low or DNA is damaged, the cell can stall here permanently and enter G0. I once spent three weeks troubleshooting why a culture of fibroblasts refused to divide, only to realize the serum concentration in the media had drifted from 10 percent down to 3 percent over a month because someone left the stock bottle open. These cells were stuck in G1 with no external signal to proceed. Fixed it by changing the media and they started cycling again within two days.
S phase is synthesis. The DNA replicates. Every chromosome goes from one chromatid to two sister chromatids held together at the centromere. This is the most error-prone part of the cycle. The replication machinery has proofreading, but it is not perfect. Things like nucleotide pool imbalance or replication fork stalling can cause problems here, and the cell has damage response pathways specifically because S phase is dangerous ground. G2 is the second gap. The cell keeps growing and checks that DNA replication finished cleanly. The spindle assembly components get made during this time. If there is incomplete replication or double-strand breaks, the G2 checkpoint blocks entry into mitosis. This checkpoint is mediated largely by ATM and ATR kinases phosphorylating Chk1 and Chk2, which then inhibit CDC25 phosphatases and keep CDK1 inactive. You do not need to memorize that pathway right now, but understanding it helps explain why certain cancer drugs target checkpoint kinases. M phase is mitosis followed by cytokinesis. Prophase, prometaphase, metaphase, anaphase, telophase. The chromosomes condense, the spindle forms, chromosomes align at the metaphase plate, sister chromatids separate, and the cell splits. The whole process in a typical mammalian cell takes about an hour. The restriction point in late G1 is the real commitment step. Before that, the cell can bail. After it passes the restriction point, it is going through the cycle whether conditions stay good or not.
Here is something most textbooks gloss over. The length of each phase varies wildly depending on cell type. A fertilized egg can go through S and M in minutes with almost no growth in between. A neuron in G0 never divides again. A stem cell in the gut crypt might complete a full cycle in eight hours. A liver cell might take over a year. The steps are the same, but the timing tells you what the cell is trying to do. Cyclins and cyclin-dependent kinases drive the transitions. Cyclin D and CDK4/6 push you through G1. Cyclin E and CDK2 trigger the G1 to S transition. Cyclin A and CDK2 run S phase. Cyclin B and CDK1 drive G2 to M. The cyclins get made, the CDKs get activated, the substrates get phosphorylated, and then the cyclins get ubiquitinated and destroyed by the proteasome so the next phase can start. It is a cascade. The destruction of cyclins is what makes the cycle go forward irreversibly. If you block the proteasome, cells get stuck in mitosis because they cannot degrade cyclin B. The spindle assembly checkpoint is another thing people get wrong. It does not just check that chromosomes are attached. It checks that they are attached to the right thing, under the right tension, and aligned at the metaphase plate. Merely being stuck to a microtubule is not enough. The checkpoint signals through MAD2 and BUBR1 to inhibit the APC/C complex until everything is properly bi-oriented. That is why drugs like taxol, which stabilize microtubules, actually trigger this checkpoint and arrest cells in mitosis. The microtubules are too stable to reorganize properly, so chromosomes never align correctly, and the checkpoint stays on indefinitely.
Get the Full Details

If you are studying this for an exam, focus on what each checkpoint monitors and what happens when it fails. G1 checkpoint monitors cell size, nutrients, DNA damage. S phase has intra-S checkpoint for replication stress. G2 checkpoint monitors DNA damage and incomplete replication. M checkpoint monitors spindle attachment. Failure at any of these leads to genomic instability, which is why these pathways are mutated in roughly half of all human cancers. But also remember that hyperactivating checkpoints can cause tissue degeneration, which is why some therapies that punch above their weight target the checkpoints rather than the DNA itself. The Rb protein is the gatekeeper at the restriction point. In its hypophosphorylated state, it binds E2F and represses transcription of S-phase genes. CDK4/6-cyclin D phosphorylates Rb, which releases E2F, which turns on genes needed for DNA replication. Growth factors stimulate cyclin D expression. No growth factor, no cyclin D, Rb stays active, cell stays in G1. This is why CDK4/6 inhibitors like palbociclib work in breast cancer. They lock Rb in its active state and starve the cell of S-phase gene expression. The biology is straightforward. The clinical application is where it gets interesting. One practical detail that matters if you ever work with this in a lab. Synchronization methods are imperfect. Serum starvation pushes cells into G0, but it also changes gene expression in ways that do not reflect normal G1. Aphidicolin blocks DNA polymerase alpha and arrests cells at the G1/S boundary, but prolonged exposure causes replication stress and DNA damage that contaminates your results. Thymidine double-block is cheaper and gentler but less precise. Pick your method based on what you are measuring, not what is easiest.
Time-lapse microscopy of individual cells has changed how we think about this. The old textbook view treats the cycle as a rigid clock. Single-cell data shows it is more stochastic. Daughter cells from the same parent can have different cycle lengths. Stress experienced in G1 can make the next S phase slower. The cycle has memory. This is probably mediated by epigenetic changes and protein dilution effects rather than anything dramatic, but it matters if you are trying to draw conclusions from population-averaged data. There is a reason the cell cycle is taught as one of the most fundamental topics in biology. Almost everything else connects to it. Development, tissue repair, cancer, aging, stem cell biology. If you understand the cycle well enough to predict what happens when a checkpoint fails or a cyclin is overexpressed, you have a framework that applies to half the problems in medicine. The parts that trip people up are usually the regulatory logic, not the phases themselves. The fact that cyclin degradation is required for progression. The fact that CDK activity needs both a cyclin and phosphorylation on the activating threonine while avoiding the inhibitory tyrosine phosphorylation. The fact that Wee1 and CDC25 are the yin and yang controlling CDK1. These are the details that separate someone who knows the steps from someone who understands the mechanism.
Why This Matters Outside a Textbook
Chemotherapy targets rapidly dividing cells because it hits S phase and M phase harder than quiescent ones. That is why hair loss and gut lining damage are common side effects. But resistance develops because tumor cells can downregulate checkpoint sensors or upregulate DNA repair, effectively smoothing over the damage that should kill them. Newer approaches try to exploit synthetic lethality. If you block the backup repair pathway in a cell that already has a broken primary one, it dies. That is how PARP inhibitors work in BRCA-mutant cancers. Understanding the steps of the cell cycle is not about passing a biology quiz. It is about having the right mental model for how living systems regulate themselves. The logic is elegant. The failures are messy. The applications are everywhere.