Why Most People Flunk This Topic
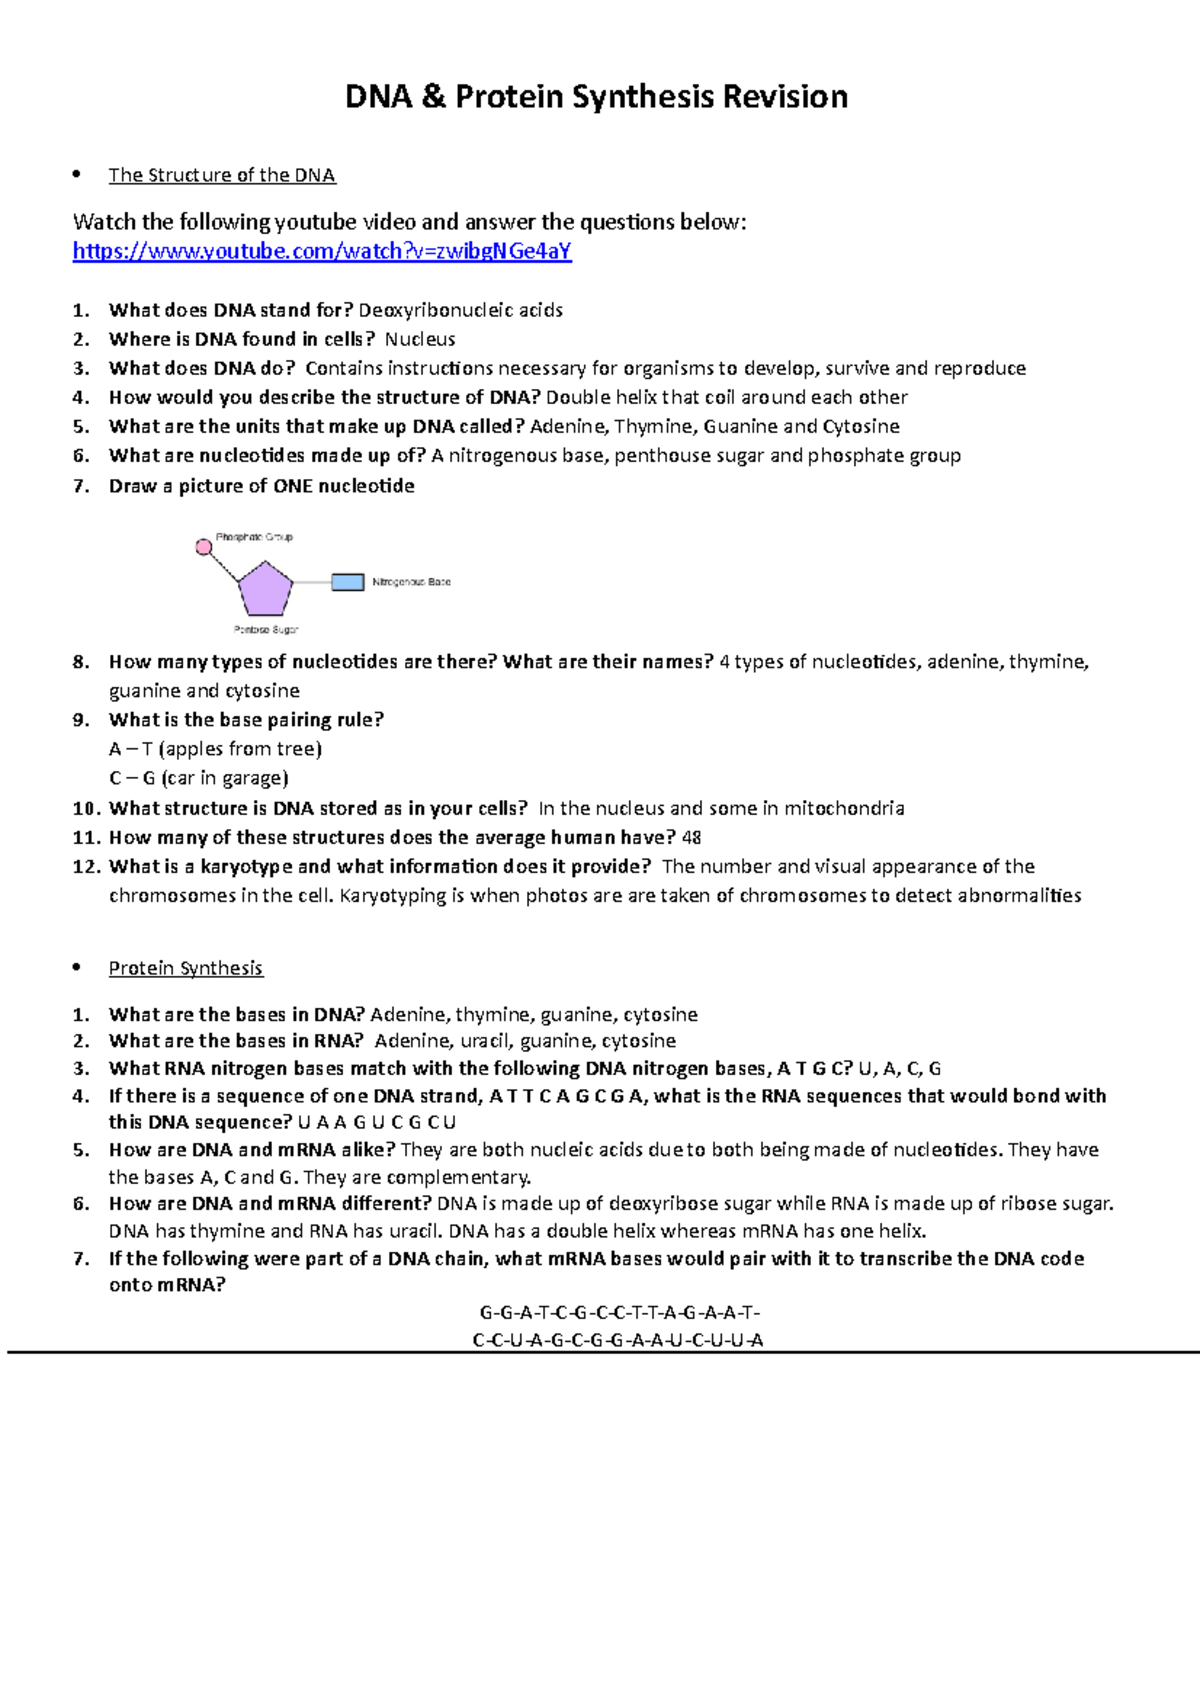
I have watched students memorize the central dogma until they could recite it backwards, then fail the first question that asked them to apply it to an actual scenario. The problem is not that the material is hard. The problem is that heredity, DNA, and protein synthesis are taught as three separate chapters when they are really one continuous process. You cannot understand one without the others, and most courses don't make that connection clear early enough. When I started tutoring this stuff, I noticed a pattern. Students who scored well always connected the dots between a Punnett square prediction and what actually happens inside the nucleus during transcription. Students who struggled treated each topic as a standalone fact list. This Study Guide Heredity Dna And Protein Synthisis approach works because it forces you to see the chain rather than isolated events.
Study Guide Heredity Dna And Protein Synthisis
The Central Dogma, Actually Understood
DNA makes RNA makes protein. That is the simplest version. The reality is messier. Reverse transcriptase exists in retroviruses. RNA can act as a catalyst without becoming protein. Non-coding RNAs regulate gene expression at multiple levels. But for an introductory course, the central dogma is still your anchor point. The thing that trips people up is not the flow of information. It is the molecular mechanics of how that flow actually happens step by step. Let me walk through it the way I explain it now after watching students miss the same details for years. DNA is double-stranded and antiparallel. One strand runs 5 prime to 3 prime, the other runs 3 prime to 5 prime. When transcription begins, RNA polymerase does not unzip the whole molecule. It opens a small transcription bubble, reads the template strand in the 3 prime to 5 prime direction, and builds the new RNA strand in the 5 prime to 3 prime direction. The coding strand looks like the RNA output, except thymine is replaced by uracil. That difference between template and coding strands causes confusion on every exam I have ever graded.
Transcription Details That Actually Matter
Promoters are not optional decorations. They are the landing site where RNA polymerase and general transcription factors bind to start transcription. In eukaryotes, the TATA box is a common promoter sequence located about twenty-five base pairs upstream from the transcription start site. Without a functional promoter, transcription does not happen regardless of how much RNA polymerase is floating around. The pre-mRNA that comes out of transcription gets processed before it ever reaches the ribosome. A five prime cap gets added to protect the transcript and help the ribosome recognize it. A poly-A tail gets added to the three prime end for stability and export efficiency. Introns get spliced out by the spliceosome, which recognizes specific sequences at exon-intron boundaries. Exons get joined back together. Alternative splicing means one gene can produce multiple different proteins depending on which exons get included. This is one of those counter-intuitive points that exams love to test and students routinely miss. I remember a student once asked me why a mutation in an intron would ever matter. The answer was straightforward once we connected it to splice site recognition. Mutations at the consensus sequences where the spliceosome binds can cause introns to be retained or exons to be skipped, producing a completely different protein product from the same gene.
Get the Full Details

Translation, or How RNA Becomes a Real Molecule
Messenger RNA leaves the nucleus and finds a ribosome. Transfer RNAs bring amino acids to the ribosome. Each tRNA has an anticodon that base-pairs with a specific codon on the mRNA. The ribosome has three sites: the A site for incoming aminoacyl-tRNAs, the P site for peptidyl-tRNAs holding the growing chain, and the E site where empty tRNAs exit. Translation starts at the start codon, usually AUG, which codes for methionine. The ribosome reads the mRNA in groups of three nucleotides. Each codon specifies one amino acid. The process continues through elongation until a stop codon appears. Stop codons do not code for any amino acid. Release factors bind to them instead, triggering the ribosome to disassemble and release the finished polypeptide. Here is a detail most study guides skip. The genetic code is degenerate. Sixty-four codons exist, but only twenty standard amino acids get specified. That means most amino acids are encoded by more than one codon. The wobble position, which is the third base in a codon, often allows a single tRNA to recognize multiple codons. This redundancy is why some mutations are silent. A change in the third position of a codon might still code for the same amino acid.
Predominant Genetic Patterns Beyond Simple Dominance
Punnett squares work fine for single-gene traits with complete dominance. Mendel's pea plants gave us that framework. Real inheritance is rarely that clean. Incomplete dominance means neither allele is fully dominant. Heterozygotes show a blended phenotype. Snapdragons with red and white alleles produce pink flowers. This is different from codominance, where both alleles express fully and simultaneously. A person with AB blood type expresses both A and B antigens on their red blood cells. These two concepts are routinely confused on tests. Multiple alleles exist when more than two allele variants are present in a population, even though any individual carries only two. ABO blood groups are the classic example. Alleles I^A, I^B, and i interact through codominance and simple dominance to produce four possible blood types.
Pleiotropy occurs when one gene influences multiple phenotypic traits. Sickle cell anemia is a textbook case. A single point mutation in the beta-globin gene causes misshapen red blood cells, which leads to anemia, pain crises, organ damage, and increased resistance to malaria. One gene, many effects.

Chromosomal Inheritance and Linkage
Genes located on the same chromosome tend to be inherited together. This is linkage. Thomas Hunt Morgan discovered this while working with fruit flies. Genes that are far apart on the same chromosome can still be separated by crossing over during meiosis I. The frequency of recombination between two genes correlates with their physical distance. Geneticists use recombination frequencies to map gene positions on chromosomes. Sex-linked inheritance follows a different pattern because the X and Y chromosomes carry different genes. Most sex-linked traits are X-linked. Males have only one X chromosome, so they express whatever allele is on that single X. Females have two X chromosomes and can be carriers without showing the trait. Red-green color blindness and hemophilia are X-linked recessive conditions. The inheritance patterns produce very different probability outcomes depending on which parent carries the allele. I once had a student fail a problem involving a carrier mother and an affected father. She kept applying autosomal recessive logic and got the Punnett square wrong every time. The fix was simply drawing the sex chromosomes explicitly instead of treating them like any other pair. Once the X and Y were labeled clearly, the genotypes fell into place.
Mutations, Their Types, and Their Consequences
A point mutation changes a single nucleotide pair. It can be a substitution, where one base is replaced by another. It can also be a frameshift, where a base is inserted or deleted. Frameshift mutations are usually more severe because they shift the reading frame of every downstream codon. Substitutions have three possible outcomes. A missense mutation changes one amino acid to another. A nonsense mutation creates a premature stop codon, producing a truncated protein. A silent mutation changes the nucleotide sequence without changing the amino acid sequence due to codon degeneracy. Chromosomal mutations involve larger structural changes. Deletions remove a segment. Duplications repeat a segment. Inversions flip a segment within the chromosome. Translocations move a segment to a different chromosome. These changes can disrupt gene function or create entirely new gene combinations.
How to Actually Study This Material
Flashcards for vocabulary are necessary but insufficient. Memorizing that transcription happens in the nucleus and translation happens in the cytoplasm tells you nothing about how those processes connect to inheritance patterns. The most effective approach is to work through full problems from start to finish. Draw the DNA sequence. Transcribe it to mRNA. Translate it to amino acids. Then introduce a mutation and trace its effect through the entire chain. This method takes longer than rote memorization initially, but it builds the kind of understanding that survives exam questions with unfamiliar scenarios. The first time I tried this, it took me about twenty minutes to work through a single ten-codon sequence. After a week of practice, I was doing the same problem in about four minutes. The speed came from pattern recognition, not from skipping steps. Pedigree analysis requires practice with actual problems. Start with simple autosomal recessive patterns and build up to X-linked and incomplete dominance cases. Draw the genotypes under each individual in the pedigree before calculating probabilities. Skipping that step causes errors every time.
What This Study Approach Does Not Handle Well
This material is foundational, not complete. It does not cover epigenetics, gene regulation through operons in bacteria, RNA interference, or the more complex quantitative trait inheritance that appears in advanced courses. If you are preparing for an AP Biology exam or a college genetics course, you will need additional resources beyond this scope. The biggest limitation is that heredity and molecular biology have advanced significantly since the standard curriculum was written. Concepts like CRISPR gene editing, CRISPR-Cas systems, and modern genomic techniques are rarely included in introductory study materials but appear frequently on competitive exams. Supplementing this guide with current reading on those topics would close that gap. Another honest limitation is that practice problems in most textbooks are generated from a narrow pool of scenarios. Real exam questions sometimes combine inheritance patterns with molecular mechanisms in ways that standard problem sets do not anticipate. Working through past exam papers and understanding the underlying logic rather than memorizing answers is the only reliable way to handle unexpected question formats.