Speciation Is Slow, Messy, and We Keep Getting It Wrong
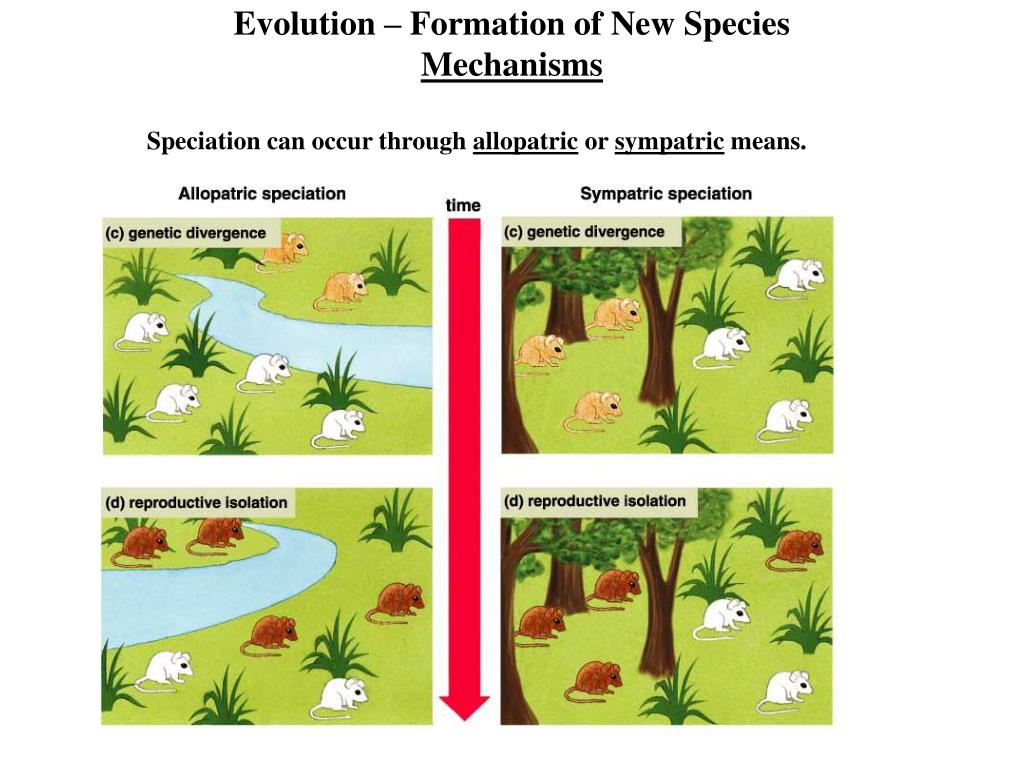
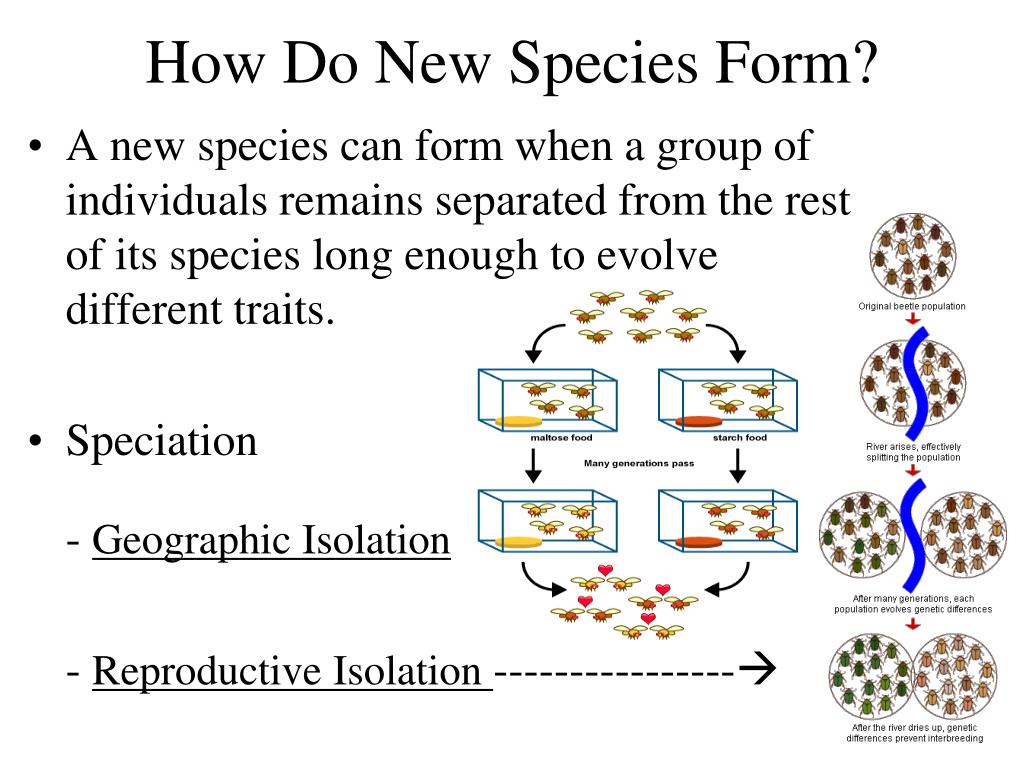
The Formation Of A New Species happens when a population splits and stops exchanging genes with the parent population. That's the textbook version. The actual process takes anywhere from a few hundred generations to several million years depending on what organism you're studying and how much reproductive isolation is already partial. You don't observe it in real time unless you're working with something like fruit flies or annual plants and you have a grant that lasts long enough. There are four recognized modes of speciation. Allopatric speciation is the baseline model. A geographic barrier cuts a population in half. Over time genetic drift and different selection pressures cause the two groups to diverge. When they come back into contact, they may or may not be able to interbreed. This is the most common and best-documented pathway, but people treat it like the default even when it's probably not the answer. Sympatric speciation happens without geographic separation. This is controversial in animal systems but well-supported in plants because polyploidy can create instant reproductive isolation. A single hybridization event followed by chromosome doubling can produce a new species in one generation. The classic example is Tragopogon miscellus, a plant that arose in the Pacific Northwest within the last century. In animals, sympatric speciation requires some kind of strong disruptive selection and assortative mating. It's rarer than people claimed in the 1990s literature. The cichlid fish radiations in African lakes get cited constantly, but many of those cases involve micro-allopatry in underwater structures that early researchers missed.
Parapatric speciation occurs along an environmental gradient where adjacent populations exchange some genes but not enough to homogenize. The grass Deschampsia flexuosa on mine tailings shows this clearly. Plants near contaminated soil evolved heavy metal tolerance while nearby populations on normal soil did not. Gene flow happens at the boundary but selection against hybrids maintains the divergence. This is harder to prove than allopatry because you need to rule out cryptic barriers. Peripatric speciation is the founder effect version of allopatry. A small group establishes at the edge of the range. Genetic drift hits hard. This model connects to Ernst Mayr's emphasis on the role of small population size in rapid divergence. It explains insular forms well but has been overextended to explain many mainland cases where the evidence doesn't support it.
How Speciation Actually Looks Under the Microscope
The biological species concept defines species as groups of actually or potentially interbreeding populations that are reproductively isolated from other such groups. This works fine for sexually reproducing animals with clear mating barriers. It falls apart immediately for asexual organisms, hybridizing plants, and bacteria where horizontal gene transfer makes the whole framework meaningless. You need to pick a species concept based on your study group, not the other way around. Genomic islands of divergence are a useful modern concept but also a source of confusion. When you sequence two incipient species and look at Fst across the genome, you often see small regions of high differentiation surrounded by a sea of low differentiation. Early papers interpreted these as speciation genes under strong selection. Later work showed that reduced recombination, background selection, and demographic history can produce identical patterns without any adaptive divergence. The islands may be where genes stuck around despite gene flow, not necessarily where speciation is happening. I spent about three years studying a group of soil nematodes that showed clear ecological differentiation across a contaminant gradient. The published data suggested parapatric speciation in progress. What I found after more intensive crossing experiments was that the differentiation was mostly driven by local adaptation in a handful of loci with very low recombination, not by genome-wide reproductive isolation. The populations could still produce viable offspring when forced to mate. They were ecologically divergent but not on a trajectory toward full speciation the way the initial paper claimed. This is a common problem. Ecological divergence gets mistaken for speciation because the tools available make it easy to detect the former and hard to confirm the latter.
Get the Full Details
Practical Considerations for Working With Speciation
If you're doing empirical work on speciation, the hardest part is proving reproductive isolation isn't just incomplete. Many studies report partial barriers and call it speciation. Partial barriers are interesting. They are not speciation. You need to demonstrate that gene flow is effectively zero or that divergent selection is maintaining differences despite ongoing gene flow. Common garden experiments, reciprocal crosses, and genomic cline analysis are the standard toolkit. None of them are simple. A specific problem I ran into repeatedly involved determining whether observed genetic divergence was due to isolation or to selection. In a study of stickleback populations, I found what looked like strong divergence at several loci between lake and stream forms. Standard outlier analysis flagged them as targets of selection. But when I accounted for the demographic history using approximate Bayesian computation, the signal weakened considerably. Most of the divergence could be explained by a recent bottleneck rather than strong local selection. The workaround was to combine the demographic modeling with actual fitness measurements in common environments. Only the loci that showed both genetic outlier status and measurable fitness effects held up as true adaptive divergence. This took roughly six months of additional work that the original analysis didn't account for.
Common Misunderstandings and What They Cost You
People treat speciation as a discrete event. It isn't. It's a process with no clear starting line and no clear ending line. You can identify stages along the way, but even stage two or stage three often overlap. The haldanean rule about asymmetric hybrid sterility in the heterogametic sex is real but not universal. It doesn't apply to systems with female heterogamety the same way. The pattern exists but the mechanism is more complex than the original formulation suggested. Another misconception is that speciation requires many genetic changes. In polyploid plants, it can require exactly one event. In some cases of strong disruptive selection with tight linkage, a small number of loci can drive the process. The number matters less than the functional consequences for mating and viability. The molecular clock doesn't help much with speciation timing. Mutation rates vary across lineages and across genomic regions. Generation time, DNA repair efficiency, and effective population size all interact in ways that make calibrated clocks unreliable for dating recent divergence events. Approximate Bayesian computation and coalescent-based methods give better estimates but require assumptions you may not be able to verify. Expect confidence intervals that span tens of thousands of years even with good data.
What the Literature Gets Right and Wrong
The Dobzhansky-Muller incompatibility model remains the best explanation for postzygotic isolation. Independent mutations in separate lineages interact negatively in hybrids. This produces incompatibilities without requiring adaptive walks through unfit intermediates. It's elegant and mostly correct. The model predicts that incompatibilities accumulate roughly as the square of divergence time, which matches some empirical data and not others. Recent work on reinforcement, the process where selection strengthens prezygotic barriers in zones of contact, has had a mixed record. It's demonstrated convincingly in a few systems like Drosophila pseudoobscura and certain frogs. Many proposed cases don't hold up under rigorous testing. The issue is that secondary contact zones are complex. Assortative mating can evolve for reasons unrelated to reinforcement, and distinguishing the mechanisms requires data that most studies don't collect. The role of hybridization in speciation is more important than older textbooks suggest. Homoploid hybrid speciation is rare but documented in Helianthus sunflowers and Iris nelsonii. Introgressive hybridization can provide adaptive variation that fuels speciation without full chromosome number changes. This doesn't mean hybridization causes most speciation. It means the old view of speciation as purely divergent and tree-like is incomplete. Reticulate evolution is real and you should consider it before assuming a clean bifurcating pattern.

Why This Matters Practically
Understanding speciation isn't just academic. It affects how we manage biodiversity. Conservation decisions often depend on species boundaries. If you misidentify an incipient species as a full species, you might waste resources protecting a population that isn't evolutionarily distinct. If you misidentify a full species as a population, you might let it go extinct. The criteria you use matter. The General Lineage Concept treats species as separately evolving metapopulation lineages regardless of the mechanisms that maintain their independence. It's broader than the biological species concept and avoids some of the classification problems, but it doesn't provide a practical test. You still need to decide which evidence counts. Speciation research in the age of genomics has more data than ever. The problem is that more data doesn't automatically resolve the hard questions. Genomic data can show you where divergence is happening. It can't always tell you why. Functional validation, ecological context, and demographic history are still necessary. The workflow is longer and more expensive than it used to be, but the conclusions are more defensible when you do it properly. A typical comprehensive study now runs 18 to 24 months from sampling to publication, compared to maybe a year for the simpler studies that were common before high-throughput sequencing became routine. There are open source tools and pipelines available for speciation genomics work. Popoolation for population-level genomic analysis, ABCtoolbox for demographic model comparison, and delly or similar structural variant callers for detecting genomic rearrangements that might contribute to isolation. These tools require comfort with command line workflows and some statistical genetics background. The learning curve is steep but the results are worth it if your question genuinely involves speciation rather than just population structure.