Speciation Doesn't Work The Way Textbooks Make It Sound
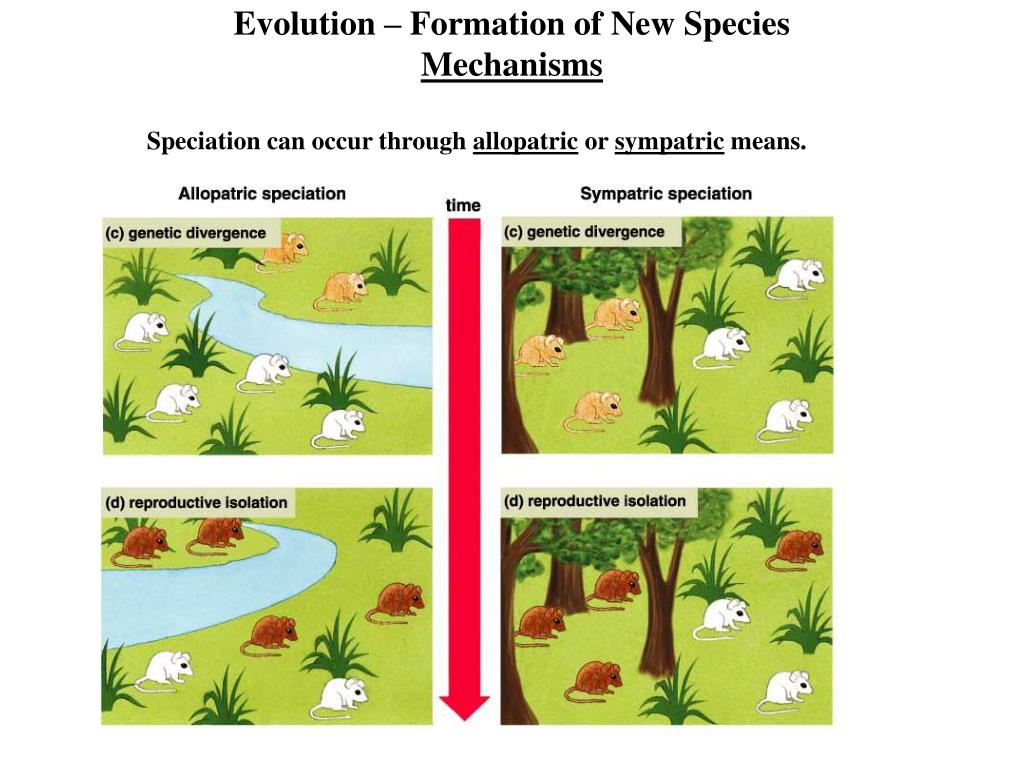
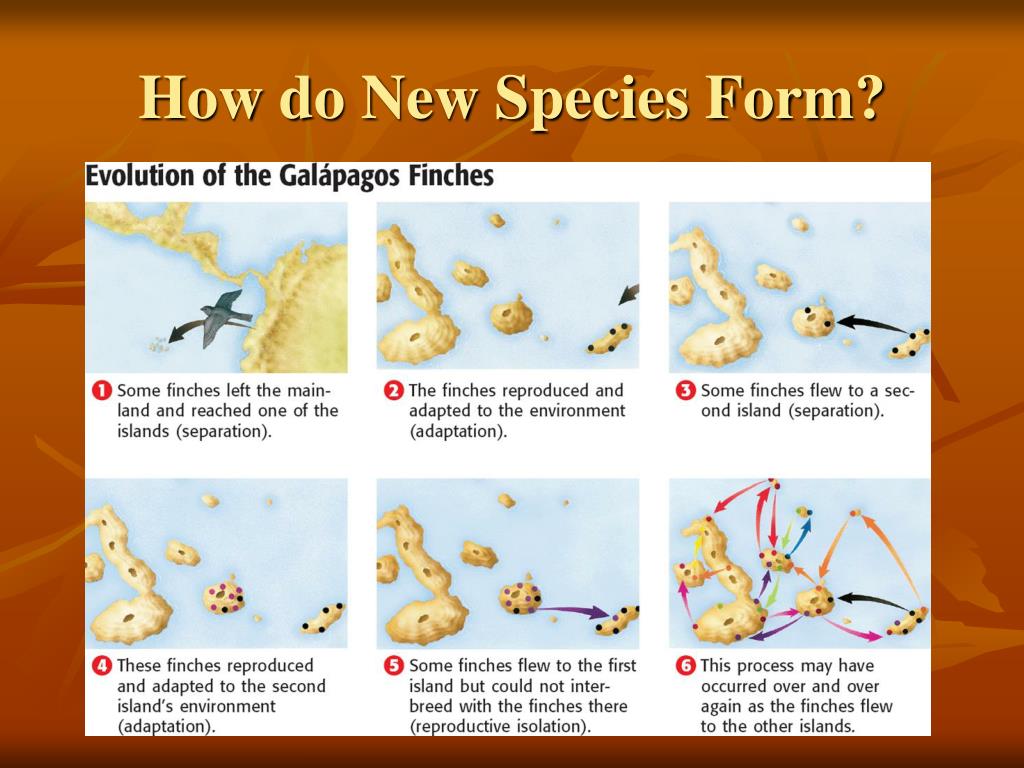
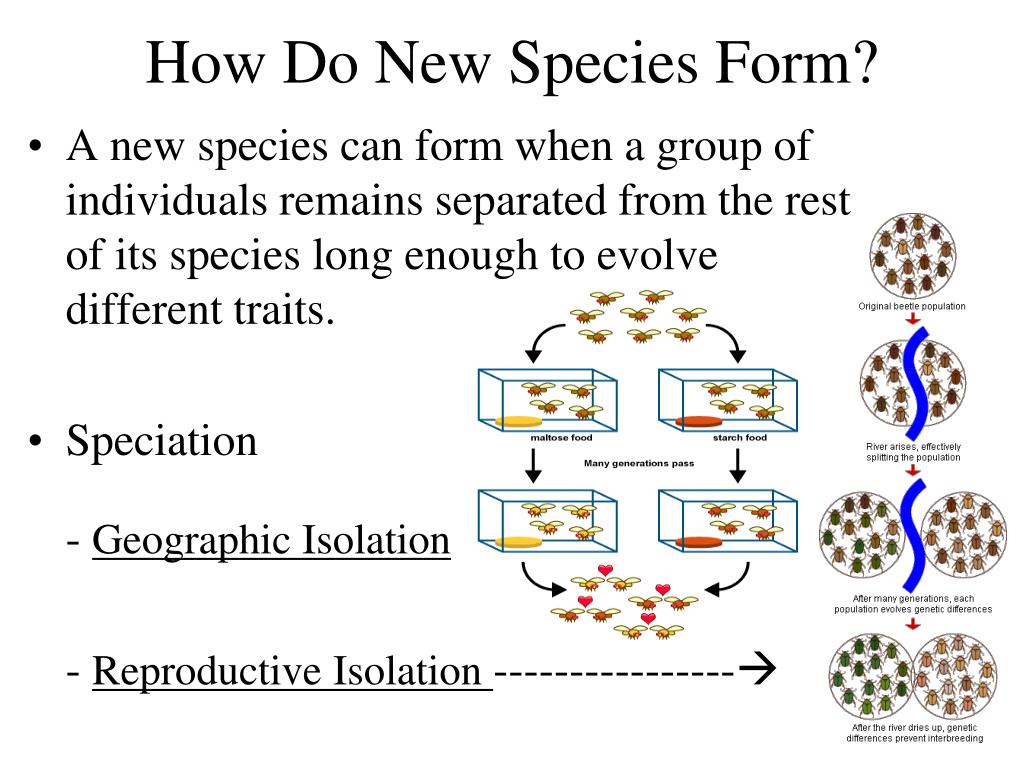
The Formation Of New And Distinct Species Through Evolutionary Processes is something people simplify into neat diagrams of branching trees, but anyone who has actually looked at species boundaries in the field knows it is messier than that. Speciation isn't a single event. It is a slow grinding process of genetic divergence that occasionally snaps into something you can recognize as a new species. The question isn't really whether it happens, it is how you know when to call it done. At its core, speciation requires reproductive isolation. Not the romantic kind. I mean physical, behavioral, or genetic barriers that prevent two populations from exchanging genes. When gene flow stops, the populations start drifting apart. Mutations accumulate independently. Natural selection pushes them in different directions if their environments differ. Over enough generations, they become so genetically distinct that even if you put them back together, they can't interbreed anymore. That is the standard model, and it is basically correct, but the details matter more than the headline. There are different pathways. Allopatric speciation happens when a physical barrier splits a population. A mountain range rises. A river changes course. A few individuals colonize an island. The separated groups evolve separately. Sympatric speciation occurs without geographic isolation, usually driven by ecological niche differentiation or polyploidy in plants. Parapatric speciation sits somewhere in between, where adjacent populations diverge despite some ongoing contact along a hybrid zone. Each pathway leaves different genetic signatures, which is how you figure out what happened after the fact.
I spent years studying cichlid fish in East African lakes, and the patterns there completely broke my initial assumptions. These fish speciated in sympatry, right alongside each other in the same water column, which shouldn't be theoretically stable for very long. Gene flow should homogenize them. What actually happened is that sexual selection combined with feeding morphology created strong assortative mating. Females preferred males of their own color pattern and jaw type. The gene flow didn't stop completely, but it was restricted enough for divergence to proceed. This is one of those cases where the textbook model is directionally right but misses the actual mechanism by a wide margin.
The Genetic Mechanics Behind Divergence
When populations separate, the first thing that happens is neutral genetic drift. Every generation, allele frequencies shift slightly due to sampling error. In small populations this is fast. In large populations it is slow. The rate matters because it determines how quickly you can detect divergence using molecular markers. Most researchers use mitochondrial DNA or microsatellites as proxies, but these don't tell the whole story. Neutral markers show you when gene flow stopped, not when reproductive isolation actually completed. Selection is what does the real work on adaptive traits. If two populations face different selective pressures, alleles conferring fitness advantages in one environment can become maladaptive in the other. This creates divergent selection. The stronger the selection and the weaker the gene flow, the faster divergence proceeds. There is a critical threshold where selection overpowers gene flow, and beyond that point, divergence accelerates non-linearly. You can model this with simple equations involving selection coefficients and migration rates, but the real world adds layers of complexity like epistasis, pleiotropy, and varying recombination rates across the genome. Genomic islands of divergence are one of those counter-intuitive findings that changed how people think about speciation. Instead of the whole genome diverging uniformly, you often see small regions of high differentiation surrounded by areas of relative similarity. These islands contain the genes responsible for reproductive isolation or local adaptation. The rest of the genome stays relatively undifferentiated because occasional gene flow still washes through. This means speciation is heterogeneous across the genome, not a blanket process. It also means you can be looking at two populations that are clearly on different trajectories while most of their DNA looks almost identical.
Get the Full Details
Another thing people miss is that hybrid zones don't always collapse. Sometimes they persist for long periods as stable boundaries between incipient species. I worked on a salamander hybrid zone in the Appalachians that had been stable for roughly forty thousand years according to molecular clock estimates. The hybrids had reduced fitness compared to purebreds, but not enough to eliminate them entirely. Gene flow continued at low levels across the zone while the two sides maintained their distinct identities. This challenges the idea that speciation is a clean binary process. It is more accurate to think of it as a continuum with fuzzy endpoints.
How To Actually Detect And Verify Speciation
The practical work involves several steps. First, you need population-level sampling. Ten individuals per population minimum, spread across the geographic range. More is better. Then you sequence. RAD sequencing or whole genome resequencing depending on budget. You want enough markers to distinguish population structure from individual variation. Structure analysis, principal component analysis, and phylogenetic network methods give you the first picture of whether groups are actually diverging. Next comes the reproductive isolation assessment. This is the part that most people skip because it is labor intensive. You do cross-breeding experiments if possible, or observe mating behavior in the field. In cichlids, we used playback experiments with recorded male courtship displays combined with color manipulation to test female mate choice. The results showed strong preference for conspecific signals within each ecological morph. That behavioral isolation was the smoking gun, even though the fish could technically produce fertile offspring in the lab. Genomic analysis follows. You calculate Fst values between populations, look for outlier loci under selection, and estimate contemporary gene flow using programs like MIGRATE or BayesAss. The key metric isNm, the number of migrants per generation. When Nm drops below one, populations are effectively isolated from a genetic standpoint. But remember, one doesn't equal complete reproductive isolation. It just means drift and selection are free to act without being swamped by gene flow.
Here is where I ran into a real problem that took me months to solve. We were studying what looked like three distinct species of snapping shrimp on opposite sides of the Isthmus of Panama. The morphological differences were clear, the genetic distances were substantial, and the geographic separation was obvious. Standard analysis said speciation was complete. Then we did functional crosses and found that the supposed "species" on the same side of the isthmus were actually more genetically similar to each other than to their counterparts on the other side. What we thought was one speciation event turning into three species was actually two independent allopatric splits followed by secondary contact and incomplete lineage sorting. The genetic data supported three groups, but the evolutionary history was far more complicated. The workaround was adding ancient DNA from museum specimens and using coalescent-based species tree methods instead of simple distance metrics. That resolved the topology correctly and showed the actual sequence of divergence events.
Common Pitfalls And Where The Model Breaks Down
The biggest mistake researchers make is equating genetic divergence with speciation. Just because two populations are genetically distinct doesn't mean they are separate species. The Biological Species Concept requires reproductive isolation, but that concept fails completely in asexual organisms, hybridizing plants, and many bacterial lineages. Even among sexually reproducing organisms, the threshold for what counts as "cannot interbreed" is arbitrary. Some supposedly distinct species hybridize readily when given the chance, while some populations within a single species show near-complete reproductive isolation in certain contexts. Polyploidy is another case that doesn't fit neat models. In plants, genome duplication can create instant reproductive isolation in a single generation. This is speciation without gradual divergence, and it accounts for maybe ten percent of speciation events in angiosperms. It is common enough that you have to consider it, but most introductory courses barely mention it. The incomplete lineage sorting problem affects phylogenetic inference across many taxa. When divergence events happen in quick succession, ancestral polymorphisms persist through multiple speciation events, creating gene trees that conflict with the species tree. This is especially problematic in rapid radiations like Darwin's finches or Hawaiian silverswords. You can get strong support for wrong topologies if you aren't careful. The workaround is using multiple unlinked loci and coalescent methods that account for ancestral variation, but this requires more data and more computational resources than standard approaches.
Time is another factor that people underestimate. Speciation typically takes tens to hundreds of thousands of generations in vertebrates. In organisms with short generation times like bacteria or fruit flies, it can happen in decades under strong selection. But in large mammals, the process is glacial. We often mistake standing genetic variation and local adaptation for early speciation when nothing has actually happened yet. The populations might be diverging, but they are just as likely to merge back together if the barrier is removed. Without demonstrating completed reproductive isolation, you are observing evolution, not speciation. Environmental change can also reverse the process. If a barrier that maintained isolation disappears, previously diverged populations can fuse back into a single gene pool. This retrogressive speciation is rare but documented in several fish and insect systems. It means that speciation is not always irreversible, which complicates any attempt to categorize it as a clean stepwise process. The formation of new species is a tendency, not a guaranteed outcome, and the outcome depends heavily on whether isolating mechanisms hold under changing conditions. The best approach combines multiple lines of evidence rather than relying on any single metric. Morphology, genetics, ecology, behavior, and geography should all be considered together. No single dataset tells the whole story, and the gaps between datasets are often where the interesting biology hides.