Understanding Sexual Reproduction in Practice
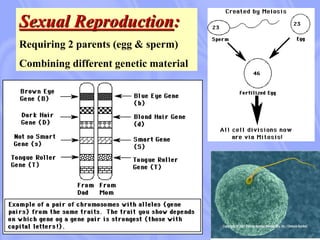
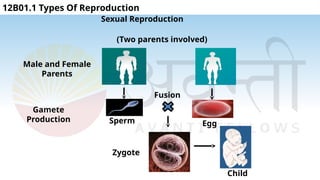
It is the most straightforward biological concept that most people casually misunderstand. Sexual reproduction involves the fusion of two specialized cells from different parents, each contributing half their genetic material. The resulting organism carries a mixed set of instructions. You cannot skip the two-parent requirement without fundamentally changing what the process is. Sexual reproduction. It has been called many things over the years, but the terminology stays consistent across biology textbooks. The core mechanism is meiosis producing haploid gametes, followed by fertilization restoring the diploid state. That is the entire skeleton of it. Everything else is variation on that theme across different organisms. When I first worked with fruit flies in a lab setting, I quickly learned that the textbook description leaves out most of the practical friction. Mating chambers need temperature control around 25°C. If you go even a few degrees off, the development timeline shifts and you lose track of generation counts. I spent three weeks trying to figure out why my cross was not producing offspring before realizing the incubator had been cycling between 23 and 27 without anyone noticing. The eggs were still forming, just far more slowly than expected, and they were degrading before hatching.
The workaround was simple once identified: mark the plates with a date stamp immediately after setting up the cross, and use a data logger instead of trusting the incubator display. Most people rely on the dial and assume it is accurate. It usually is not. That small habit probably saved me months of confused data. One thing beginners consistently miss is the assumption that two parents guarantees genetic diversity. That is not always true. If both parents share recent common ancestry, the offspring can end up with remarkably low heterozygosity despite the two-parent mechanism. Inbreeding depression shows up fast in organisms with short generation times. I watched a lab colony of nematodes collapse genetically within six generations because someone only maintained a small number of breeding pairs. The process itself was working perfectly. The gene pool was just too narrow. Another counter-intuitive point is that hermaphroditism complicates the whole two-parent framework. Many plants and some animals are simultaneous hermaphrodites, carrying both male and female reproductive organs. They can self-fertilize or cross-fertilize. When selfing occurs, you get an organism that functionally reproduces alone, even though the underlying cellular mechanism is still technically sexual reproduction. The classification does not change. The outcome looks very different from the outside though.
There are honest downsides to relying on sexual reproduction as your primary model. It requires finding a mate, which costs energy and time. It halves your genetic contribution to each offspring compared to asexual cloning. Every individual only passes on fifty percent of its genome rather than one hundred percent. From a pure reproductive efficiency standpoint, asexual reproduction wins on numbers every single time. The trade-off is that asexual populations accumulate deleterious mutations faster and adapt more slowly to environmental changes. That is the well-known Muller's ratchet problem. You gain diversity at the cost of speed and efficiency. If you are studying this for a class, focus on understanding meiosis stages rather than memorizing definitions. Knowing what happens during prophase I and how crossing over creates recombinant chromosomes will answer most questions better than any glossary entry. If you are working with actual organisms, keep detailed records of parentage and generation numbers. Your future self will thank you when you need to trace a trait back three generations and the notes from last month are the only thing standing between you and a broken experiment.
Get the Full Details