
So you actually need to understand the Krebs cycle for something real
I ran into this the other day when a grad student was trying to trace metabolic flux through their cell culture experiment and kept getting garbage data because they didn't actually understand what happens after pyruvate enters the mitochondria. They were measuring citrate levels and assuming they could back-calculate everything else linearly, which is a fundamental misunderstanding of how the cycle works under physiological conditions. Let me just walk through what actually matters here.
Why the name is confusing and what the thing actually does
The Krebs Citric Acid Cycle is also called the TCA cycle or the citric acid cycle. They're all the same thing. Named after Hans Krebs, who won the Nobel Prize for it, and it runs in the mitochondrial matrix of eukaryotic cells or the cytoplasm of prokaryotes. The cycle takes acetyl-CoA and oxidizes it to CO2 while generating reducing equivalents in the form of NADH and FADH2, plus one GTP (or ATP depending on the organism) per turn. That's the summary version. The actual mechanism is where things get messy and where people usually stumble. The first step is citrate synthase condensing acetyl-CoA with oxaloacetate to make citrate. This is the committed step. It's highly exergonic and essentially irreversible under physiological conditions, with a delta G of about -32 kJ/mol. If you're modeling this or trying to manipulate flux through the pathway, that irreversibility is why you can't just push the reaction backward. I've seen people try to design synthetic pathways that essentially reverse this step, and it doesn't work because the thermodynamics are genuinely unfavorable in the reverse direction without massive energy input.
Then aconitase converts citrate to isocitrate through the intermediate cis-aconitate. This is a dehydration-rehydration sequence. Aconitase contains an iron-sulfur cluster, which makes it sensitive to oxidative stress and reactive oxygen species. In practice, this means that under conditions of cellular stress, aconitase activity drops, which backs up citrate and shifts the entire metabolic state of the cell.
Get the Full Details

The three rate-limiting steps and why they matter
If you only remember three enzymes from this cycle, make it these. Isocitrate dehydrogenase, alpha-ketoglutarate dehydrogenase, and citrate synthase. These are the control points. Isocitrate dehydrogenase is allosterically activated by ADP and inhibited by ATP and NADH. This makes biological sense - when the cell has plenty of energy, the cycle slows down. When energy is low, it speeds up. But the counter-intuitive part is that this enzyme is often the primary rate-limiting step in many cell types, not citrate synthase as introductory textbooks sometimes imply. I spent a couple days troubleshooting why flux through the cycle wasn't responding to substrate availability in a cancer cell line I was working with, and it turned out the limiting factor was always isocitrate dehydrogenase activity, not substrate concentration. Adding more oxaloacetate or acetyl-CoA did nothing because the bottleneck was downstream. Alpha-ketoglutarate dehydrogenase is structurally similar to the pyruvate dehydrogenase complex and uses the same cofactors: thiamine pyrophosphate, lipoic acid, CoA, FAD, and NAD+. It's inhibited by its products - NADH and succinyl-CoA - and by high ATP. This is also a highly regulated point. The enzyme complex is particularly sensitive to reactive oxygen species because of its lipoic acid cofactor, which can be oxidized and inactivated.
Citrate synthase is inhibited by ATP, NADH, and succinyl-CoA, and by citrate itself in some organisms. In mammalian systems, it's less of a primary control point than the other two but still important for integrating signals from the energy status of the cell.
What happens in between the big steps
After isocitrate dehydrogenase produces alpha-ketoglutarate and NADH, alpha-ketoglutarate dehydrogenase produces succinyl-CoA and another NADH. Then succinyl-CoA synthetase converts succinyl-CoA to succinate while generating GTP (or ATP). This is the only substrate-level phosphorylation in the cycle. Succinate dehydrogenase then converts succinate to fumarate, reducing FAD to FADH2. This enzyme is unique because it's embedded in the inner mitochondrial membrane as part of Complex II of the electron transport chain. It's the physical link between the Krebs cycle and oxidative phosphorylation. When people talk about the connection between these two processes, this is the enzyme they're referring to. Fumarase hydrates fumarate to malate, and then malate dehydrogenase oxidizes malate back to oxaloacetate, producing the third NADH of the cycle. This last step is actually endergonic under standard conditions with a positive delta G, but it proceeds forward in the cell because the concentration of oxaloacetate is kept extremely low by its rapid consumption in the citrate synthase reaction. This is a classic example of how thermodynamic calculations based on standard conditions can mislead you about what's happening in an actual biological system.
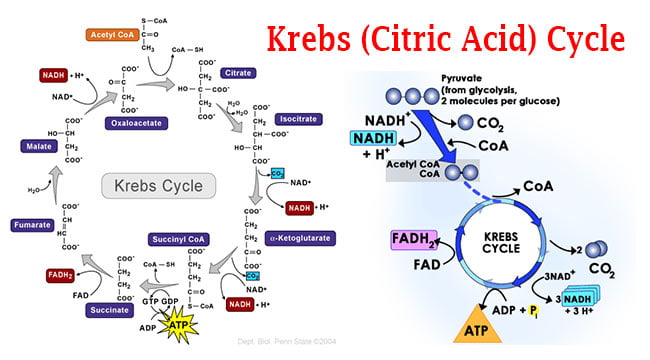
Common mistakes people make when learning The Krebs Citric Acid Cycle
The biggest one is thinking of it as a simple cycle that turns once per glucose molecule. A glucose molecule produces two pyruvate molecules, which become two acetyl-CoA molecules, so the cycle turns twice per glucose. But that's not the whole story. The oxaloacetate is regenerated, yes, but the intermediates are also siphoned off for biosynthesis. When cells need to make amino acids or heme or fatty acids, they pull intermediates out of the cycle. This is called anaplerosis when you put stuff back in, and cataplerosis when you take it out. Another mistake is thinking the cycle produces a lot of ATP directly. It produces one GTP per turn, which is roughly equivalent to one ATP. The real payoff comes from the NADH and FADH2 that feed into the electron transport chain, where each NADH generates about 2.5 ATP and each FADH2 generates about 1.5 ATP through oxidative phosphorylation. So the full yield per acetyl-CoA is about 10 ATP equivalent, and per glucose molecule (two turns of the cycle) it's about 20 ATP from the cycle's reducing equivalents plus the 2 GTP directly produced. I've also seen people confuse the NADH produced in the cycle with the NADH produced during glycolysis. Glycolysis produces NADH in the cytoplasm, and that NADH can't directly cross the mitochondrial membrane. The malate-aspartate shuttle or the glycerol-3-phosphate shuttle has to move those reducing equivalents across, and the efficiency depends on which shuttle is being used. This detail matters if you're calculating energy yields accurately.
When the cycle doesn't work the way you expect
Here's a practical problem I ran into that took me way too long to figure out. I was measuring oxygen consumption rates in isolated mitochondria from liver tissue and the respiration support looked wrong. The P/O ratio was lower than expected, and the cycle intermediates were accumulating at unusual points. I kept checking my reagent preparations and the integrity of the mitochondria, but everything looked fine. The issue turned out to be that I was using malate as a substrate without adding succinate or another source of FAD-linked oxidation. Malate alone feeds electrons into the chain only through NADH-linked complexes, and under certain conditions the NADH generated can create a bottleneck when the NAD+ pool gets depleted faster than it can be regenerated through the electron transport chain. Once I added a small amount of succinate to provide FADH2-linked input and balance the electron flow, the respiration rates normalized and the intermediate profiles made sense. It's a subtle point that almost nobody mentions in the standard protocols. Another edge case is that the cycle can run in reverse under certain conditions, particularly in photosynthetic organisms and some bacteria, to fix carbon. Even in mammals, there's evidence for reverse flux under specific metabolic states, though it's minor compared to the forward direction. If you're doing isotope tracing experiments, this reverse flux can contaminate your data if you don't account for it.
The cycle also connects to other metabolic pathways in ways that are easy to overlook. The succinyl-CoA produced in the cycle is a precursor for heme synthesis. Oxaloacetate can be converted to aspartate, which feeds into nucleotide synthesis. Alpha-ketoglutarate is a precursor for glutamate and then other amino acids. Citrate exported to the cytoplasm is the source of acetyl-CoA for fatty acid synthesis. When you're thinking about metabolism, the Krebs cycle doesn't exist in isolation - it's a hub, and perturbing any connected pathway affects it.
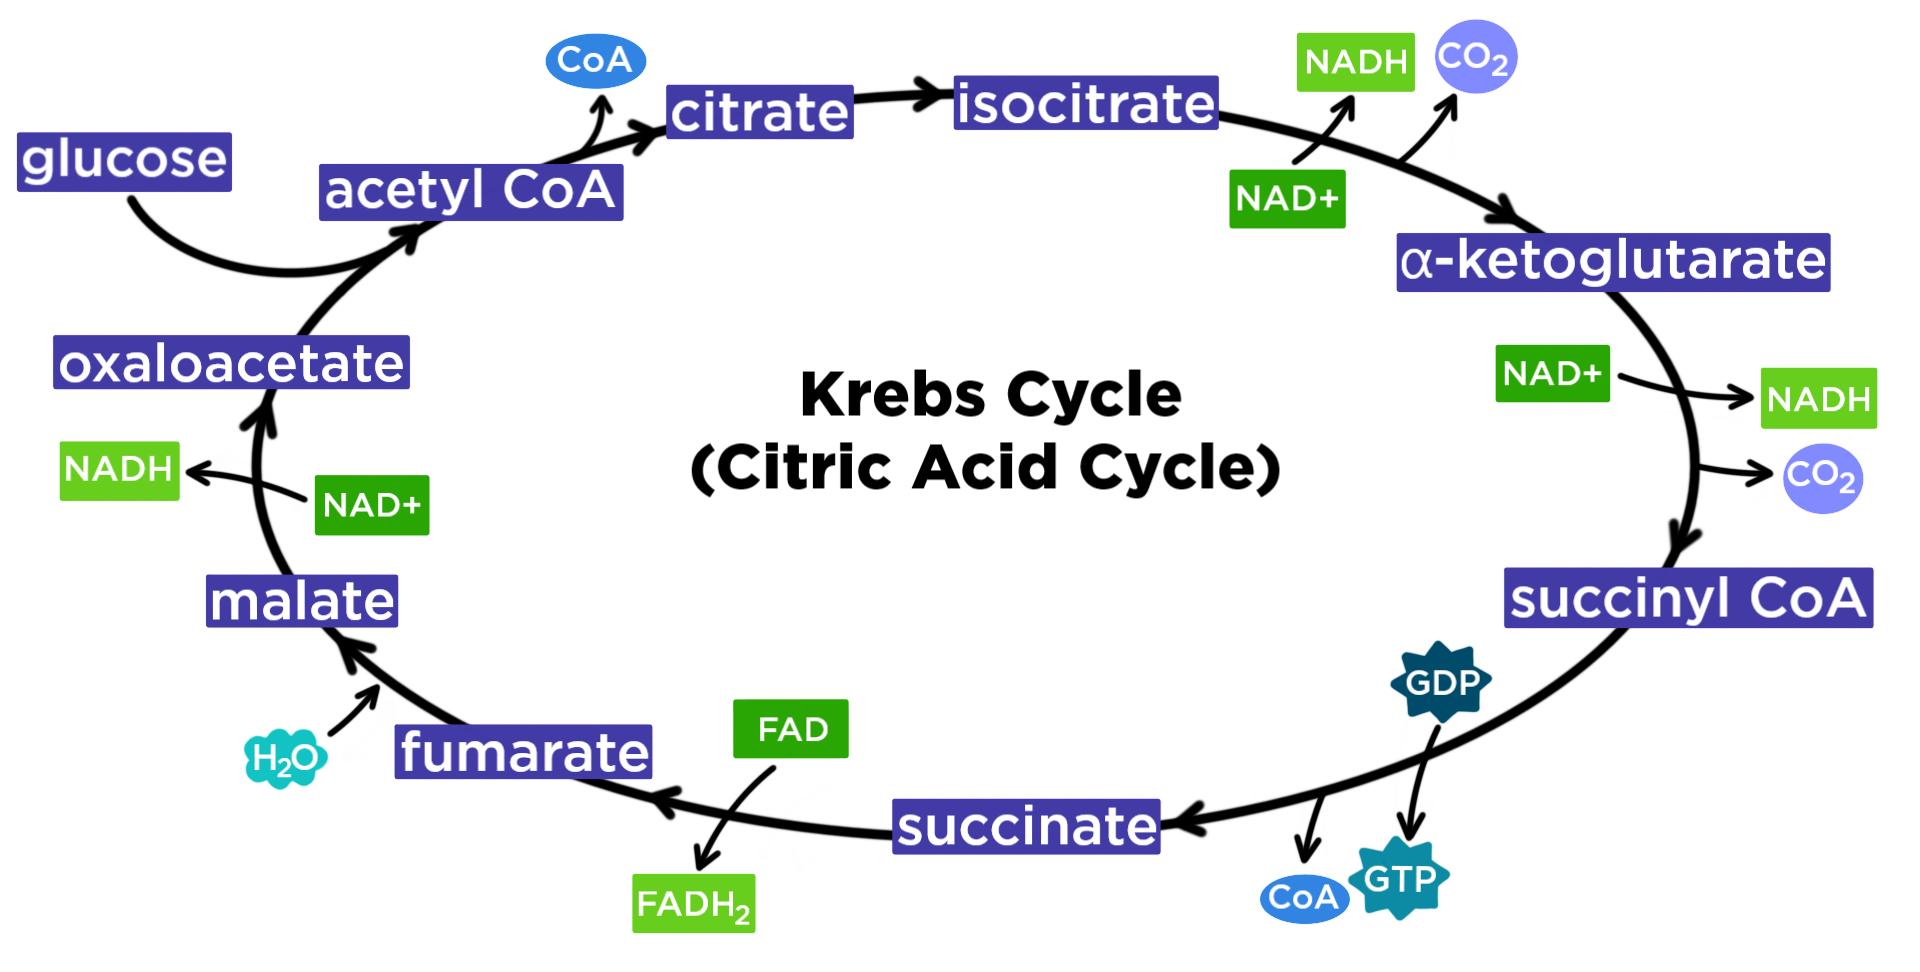
A quick reference for the actual yield
Per acetyl-CoA entering the cycle: 3 NADH (each worth about 2.5 ATP through the electron transport chain) 1 FADH2 (worth about 1.5 ATP)
1 GTP (directly equivalent to 1 ATP) 2 CO2 released Per glucose (two turns): approximately 20 ATP equivalent from the cycle reactions themselves, plus the 2 NADH from glycolysis and the 2 NADH from pyruvate dehydrogenase, bringing the total oxidative phosphorylation yield to around 30-32 ATP per glucose in eukaryotic cells.
The exact numbers vary slightly depending on the shuttle system and the organism, and some newer estimates suggest slightly lower yields than the classical textbook numbers, but this is the ballpark you should be working with. If you're studying this for an exam, focus on understanding the connectivity and regulation rather than memorizing every intermediate. The cycle is elegant but it's also heavily integrated with everything else in metabolism, and that integration is what actually matters in practice.


