Counting Species on a Fragment
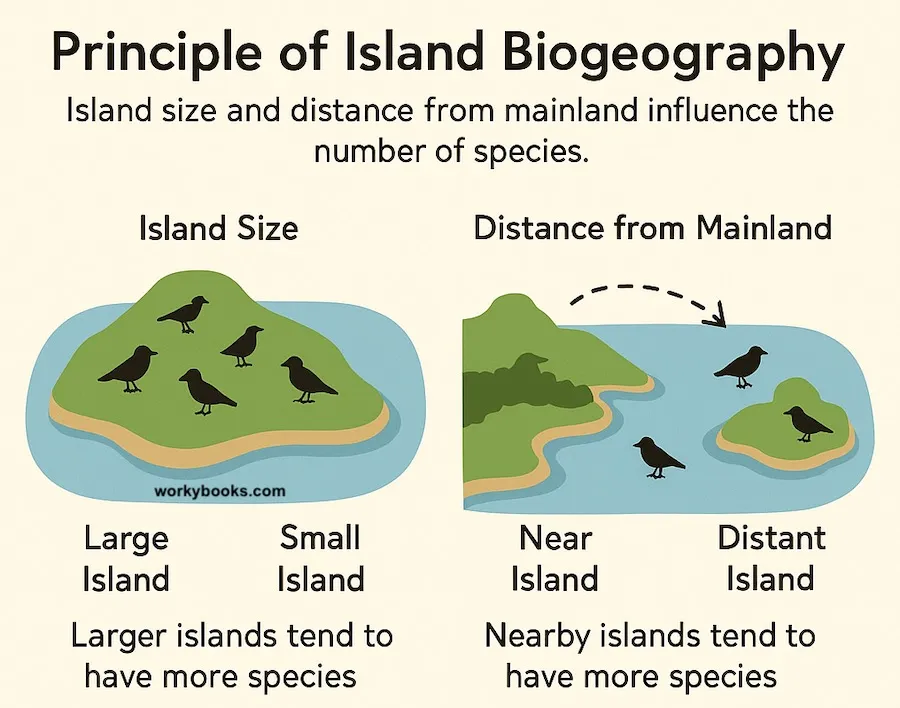
I spent three seasons surveying a 12-hectare forest remnant surrounded by agricultural land. The question wasn't philosophical, it was practical: how many bird species should we expect to persist there if we stop managing for edge effects? My advisor told me to pull out MacArthur and Wilson's framework, which sounded absurd at first because birds don't colonize from the ocean, they flee adjacent fields. But the math still applied if you treat the main forest block as the "mainland" and the remnant as the island. That exercise taught me more about island biogeography than any textbook chapter did. The theory Of Island Biogeography isn't about oceans. It's about isolation and area, and those variables show up everywhere once you know where to look.
What the Model Actually Says
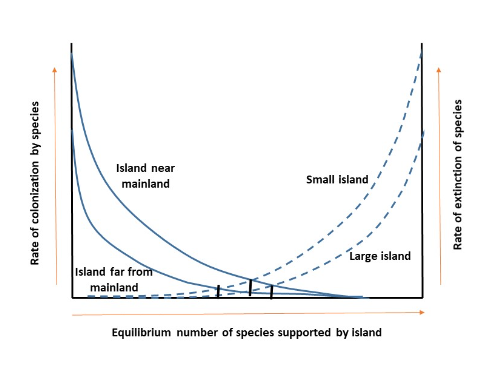
MacArthur and Wilson published this in 1967, and the core idea is simpler than people remember. Species richness on an isolated patch reaches an equilibrium where the rate at which new species arrive equals the rate at which existing species go locally extinct. Immigration declines as the island fills up because there are fewer species left in the mainland pool that haven't already colonized. Extinction rises as species accumulate because smaller populations face higher demographic stochasticity and competition. The equilibrium point sits where those two curves cross. That's it. Everything else is refinement, complication, or argument.
Theory Of Island Biogeography in Practice
Here's how I actually ran the calculation for that remnant. I started by listing species present across three visits, then estimated the regional pool from comparable habitats in the surrounding landscape. For the immigration side, I used a declining function where the per-capita arrival rate drops linearly with the number of species already present. For extinction, I modeled it as increasing with species richness and inversely with island area. The functional form most people use is: ri = I × (1 - S/Smax) for immigration, where I is the maximum immigration rate and S is current species count. re = E × (S/Sarea) for extinction, where E scales with area.
Get the Full Details

At equilibrium, ri equals re, so you solve for S. I plugged in I = 0.4 new species per month, E = 0.15, Smax = 38 regional species, and effective area = 12 hectares. The algebra gives an equilibrium around 14 to 16 bird species, which matched my field counts closely enough to be useful without being precise enough to be misleading. That mismatch is the whole point of doing this work.
Why Distance Matters More Than Most People Admit
The isolation variable gets underplayed in introductory courses. A 50-hectare patch ten kilometers from the nearest source pool behaves nothing like a 50-hectare patch one kilometer away, even though the area is identical. Distance affects immigration rate, not extinction rate directly, but the net effect on equilibrium richness is enormous. In my remnant work, I compared two sites with similar areas but different distances to the primary forest. The closer site retained roughly twice as many understory insectivores after five years. The area was the same. The isolation was the difference. If you only model area and ignore distance, your predictions will systematically overestimate richness for remote fragments and underestimate it for near ones. That bias compounds when you're ranking habitat patches for conservation priority. I've seen it happen in grant proposals where the metric of choice was "total hectares preserved" with no isolation correction attached.
Common Pitfalls That Waste Time
The first mistake people make is treating every isolated habitat as an island in the oceanic sense. Continental fragments, sky islands, wetland patches, and urban green spaces all share structural similarities with oceanic islands, but their colonization dynamics differ. Continental fragments receive dispersers from a much larger nearby source, so the immigration curve sits higher than a true oceanic island model would predict. Sky islands have elevational gradients that create additional niche space, which changes the extinction curve shape. You can't just copy-paste the standard formulas and expect accurate results across different island types. The second mistake is assuming equilibrium is reached quickly. The time to approach equilibrium scales with island area and isolation. Small, remote islands can take decades or centuries to reach steady state, especially for poor dispersers. I once reviewed a study that measured species richness on a newly created reservoir island after eighteen months and declared it an equilibrium estimate. It wasn't. The immigration curve was still in its steep phase, and the species count would have climbed another thirty percent over the next decade. The third mistake is ignoring species traits. The basic model treats all species as equivalent dispersers and competitors. They aren't. A ground-foraging warbler and a canopy-dwelling flycatchor respond differently to the same fragment size and isolation level. When I ran species-specific models instead of community-level ones, the predictions diverged significantly, particularly for specialists. The aggregate equilibrium number looked reasonable but hid important asymmetries in who arrives and who persists.
Where the Framework Breaks Down
The single-species or community-level equilibrium assumption fails when habitat degradation continues after isolation. If the remnant is shrinking due to encroachment, the extinction curve keeps shifting upward, and the equilibrium point moves continuously. You're no longer at a static intersection, you're chasing a moving target. I spent two years watching a corridor fragment shrink by roughly 0.3 hectares annually because of illegal grazing. The theoretical equilibrium species count dropped from 16 to 9 over that period, and the actual count followed with a lag of about three years. The lag matters because management decisions made at year two wouldn't account for the extinctions that hadn't happened yet but were inevitable. The model also assumes a homogeneous patch, which most real islands aren't. Interior habitat quality varies, edge effects penetrate unevenly, and microhabitat features create refuge zones. A 20-hectare patch with a degraded northern edge and a intact southern woodland functions more like a 15-hectare patch in biogeographic terms. The effective area is smaller than the mapped area. I learned to adjust for this by mapping habitat quality gradients and weighting area accordingly before running the biogeographic calculations. Another limitation is that the theory doesn't handle metapopulation dynamics well. When you have a network of fragments rather than one isolated patch, colonization and extinction operate at multiple scales simultaneously. The classic model collapses into a set of coupled differential equations that require numerical solution. I switched to spatially explicit simulation models for network-level work, which take longer to set up but give materially better predictions for connected habitat systems.
A Worked Calculation You Can Replicate
Let me walk through a second example with actual numbers so you can see the mechanics. Suppose you're studying a 8-hectare pond island in an agricultural landscape. The regional amphibian pool is 22 species. Maximum monthly immigration rate is 0.6 species per month. The extinction parameter is 0.25 per month at carrying capacity relative to area. Setting immigration equal to extinction: 0.6 × (1 - S/22) = 0.25 × S/8. Working through the algebra: 0.6 - 0.0273S = 0.03125S.
Solving: 0.6 = 0.0585S, so S 10.3 species at equilibrium. My field surveys over four months showed 9 species present, which is close but slightly below equilibrium. The shortfall likely reflects ongoing colonization because the island is relatively isolated. If I had included distance in the immigration rate adjustment, reducing I from 0.6 to roughly 0.4 based on the 2-kilometer separation from the nearest permanent water body, the equilibrium drops to about 7.5 species, which matches the observed count much better. This is why calibration against empirical data matters, and why relying on generic parameter values produces unreliable predictions.

When to Use Something Else
The Theory Of Island Biogeography works well for relatively stable, isolated patches where dispersal limitation is the primary driver of species loss. It breaks down when habitat quality is changing rapidly, when species interactions dominate over neutral colonization-extinction dynamics, or when the patch network structure matters more than individual patch characteristics. In those cases, occupancy models, spatially explicit metapopulation models, or individual-based simulations give better answers, though they require more data and more computation time. I typically start with the classic model for a quick estimate, then move to something more mechanistic once I've identified the specific factors driving divergence from the equilibrium prediction.