Working With True-Bred Lines in Practice
True breeding means a single trait stabilizes across generations because the organism is homozygous at the relevant locus. When you say true breeding, you're talking about homozygosity for the alleles you care about, not a vague promise of uniformity. The definition sounds clean. In the lab it's messier. I still remember a cross I set up in grad school where the parental line looked perfectly true-breeding for flower color for six generations, then suddenly produced a ~3% lavender fraction in the F2 after an outcross event I hadn't caught. The fix was to switch from phenotype-based selection to a simple PCR assay tracking the causal SNP, and to keep bulk seed from each selfed pod rather than relying on a handful of representative plants. You don't catch that drift by looking at a tray of flowers. You catch it by genotyping and by pooling sample lots early.
True Breeding Definition Biology
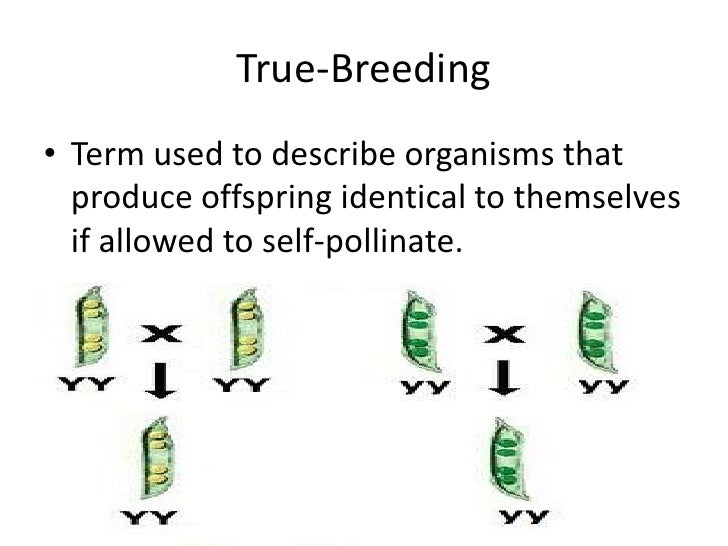
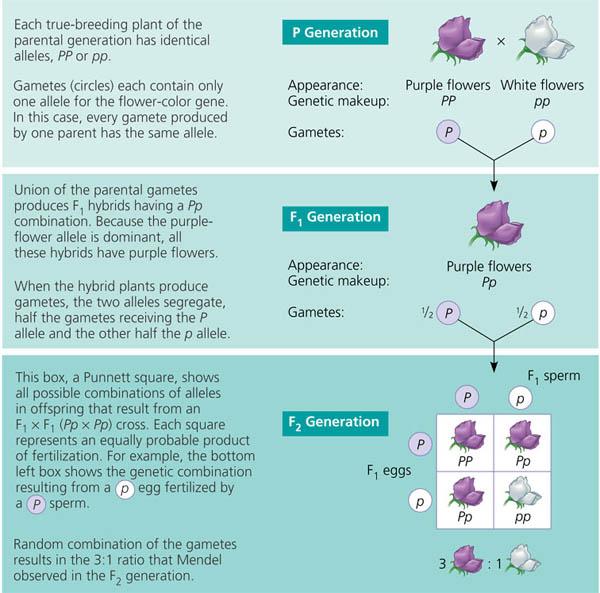
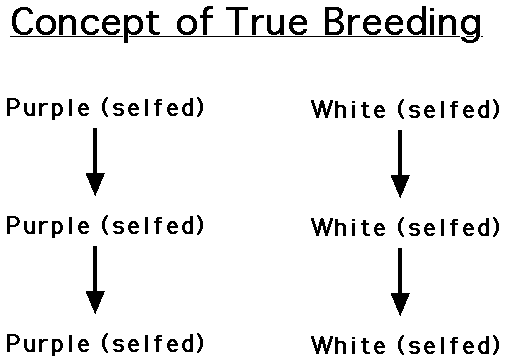
At the textbook level the true breeding definition biology is straightforward: an individual is true breeding for a trait when its progeny, produced by self-fertilization or mating with an identical genotype, consistently display the same phenotype as the parent across generations. The underlying requirement is homozygosity at the loci that determine that trait. If you self a plant that is AA at the color locus, every offspring will also be AA and show the same color. That stability is what breeders exploit when they lock in a line. The practical workflow is less about reading the definition and more about managing the probability that any given locus is still heterozygous. In a diploid starting from a heterozygous F1, each round of selfing halves the heterozygosity. After four generations of selfing, the expected heterozygosity is roughly 6.25% of the original genome-wide level, which means a typical line is near fixation at most loci, but not guaranteed. A fifth generation pushes that down to about 3%, and a sixth drops it to roughly 1.5%. Most published protocols ask for at least six to eight generations of selfing before a line is called true breeding, because the tail of heterozygous loci can linger and cause late segregation. If you're working with a dominant marker or a clearly visible recessive phenotype, the simplest verification step is a test cross. Self the candidate line and score the progeny. If every plant displays the parental phenotype across a reasonable sample size, the line is likely fixed for that allele. For a recessive trait tested at a single locus, screening 20 to 30 individuals typically gives you enough power to rule out heterozygosity with high confidence. One segregating plant in a sample of thirty strongly suggests the parent is not homozygous.
There are a few cases where phenotype scoring alone is unreliable. Incomplete penetrance can make a homozygote look like a different class. Variable expressivity can make two identical genotypes look different. Pleiotropy means fixing one trait might drag along an unwanted linked phenotype. That is why many labs pair phenotypic evaluation with molecular markers. Even a cheap SRAP or simple dominant marker panel can flag residual heterozygosity faster than waiting another generation for a phenotypic readout. Another nuance people miss is that true breeding is always trait-specific. A line can be true breeding for seed color while remaining heterozygous at a neighboring disease-resistance locus. Fixation at one locus does not imply genome-wide homozygosity, especially in outcrossing species where linkage disequilibrium decays slowly. If your goal is an inbred line, you run repeated selfing or sibling mating until you reach the desired level of homozygosity, then you validate each target trait independently rather than assuming the whole genome is locked. Speed matters here. If you self-pollinate manually, each generation takes one growing season for most annuals and often longer for perennials. You can compress timelines with rapid cycling protocols, doubled haploid production in crops like Brassica or maize, or bulk forward selection when you are building a population rather than a single line. Doubled haploids are particularly useful because they generate complete homozygosity in a single step after chromosome doubling, which avoids the long slog through multiple selfing generations. The trade-off is equipment and tissue-culture time, and not all species respond well to the induction step.
Get the Full Details
When I need to confirm a line quickly, I start with three things: a moderate sample size for phenotypic scoring, a small bulk of DNA from leaf tissue for a couple of linked markers, and a careful record of which parent contributed which allele so I can back-track if segregation appears later. Keeping a backup seed stock from each generation also prevents a contaminated batch or a missed self from erasing months of work. I once lost an entire trial when a container mislabeled in late October turned out to be from the F3 instead of the F5, and the line had already started to segregate for a trait I thought was fixed. That error cost me roughly three weeks of greenhouse time and a revised protocol where every pot gets a second label tied to the generation number and the lot ID. For organisms that do not self-fertilize easily, the approach shifts. You can use controlled sibling mating, backcrossing with a recurrent parent when the goal is to introgress a single trait, or single-seed descent to maintain diversity while gradually increasing homozygosity. Each method has a different bottleneck. Backcrossing locks in a target locus fast but retains a large portion of the donor genome elsewhere. Single-seed descent is efficient for population development but requires many generations before the average line is close to true breeding for any specific locus. One more practical detail: seed maintenance and viability. True breeding lines often lose vigor if you let seed age poorly or store at fluctuating humidity. I keep seed at a stable low moisture level and rotate stocks every few years rather than hoarding old seed indefinitely. Old seed germinates unevenly, which introduces sampling noise into your phenotype data and makes it look like segregation when the real problem is germination failure in a subset of the test batch.
The bottom line is that the concept is simple, but execution depends on sample size, generation count, and the biology of the organism. Homozygosity approaches fixation with repeated selfing, but fixation is probabilistic, not automatic. Verification by progeny testing plus a small marker panel is usually enough to catch the edge cases. When a line behaves unexpectedly, check the sample size, check the storage history, and then check the genotypes before revising the definition you are using.