Getting to Grips with Voltage Gated Ion Channels
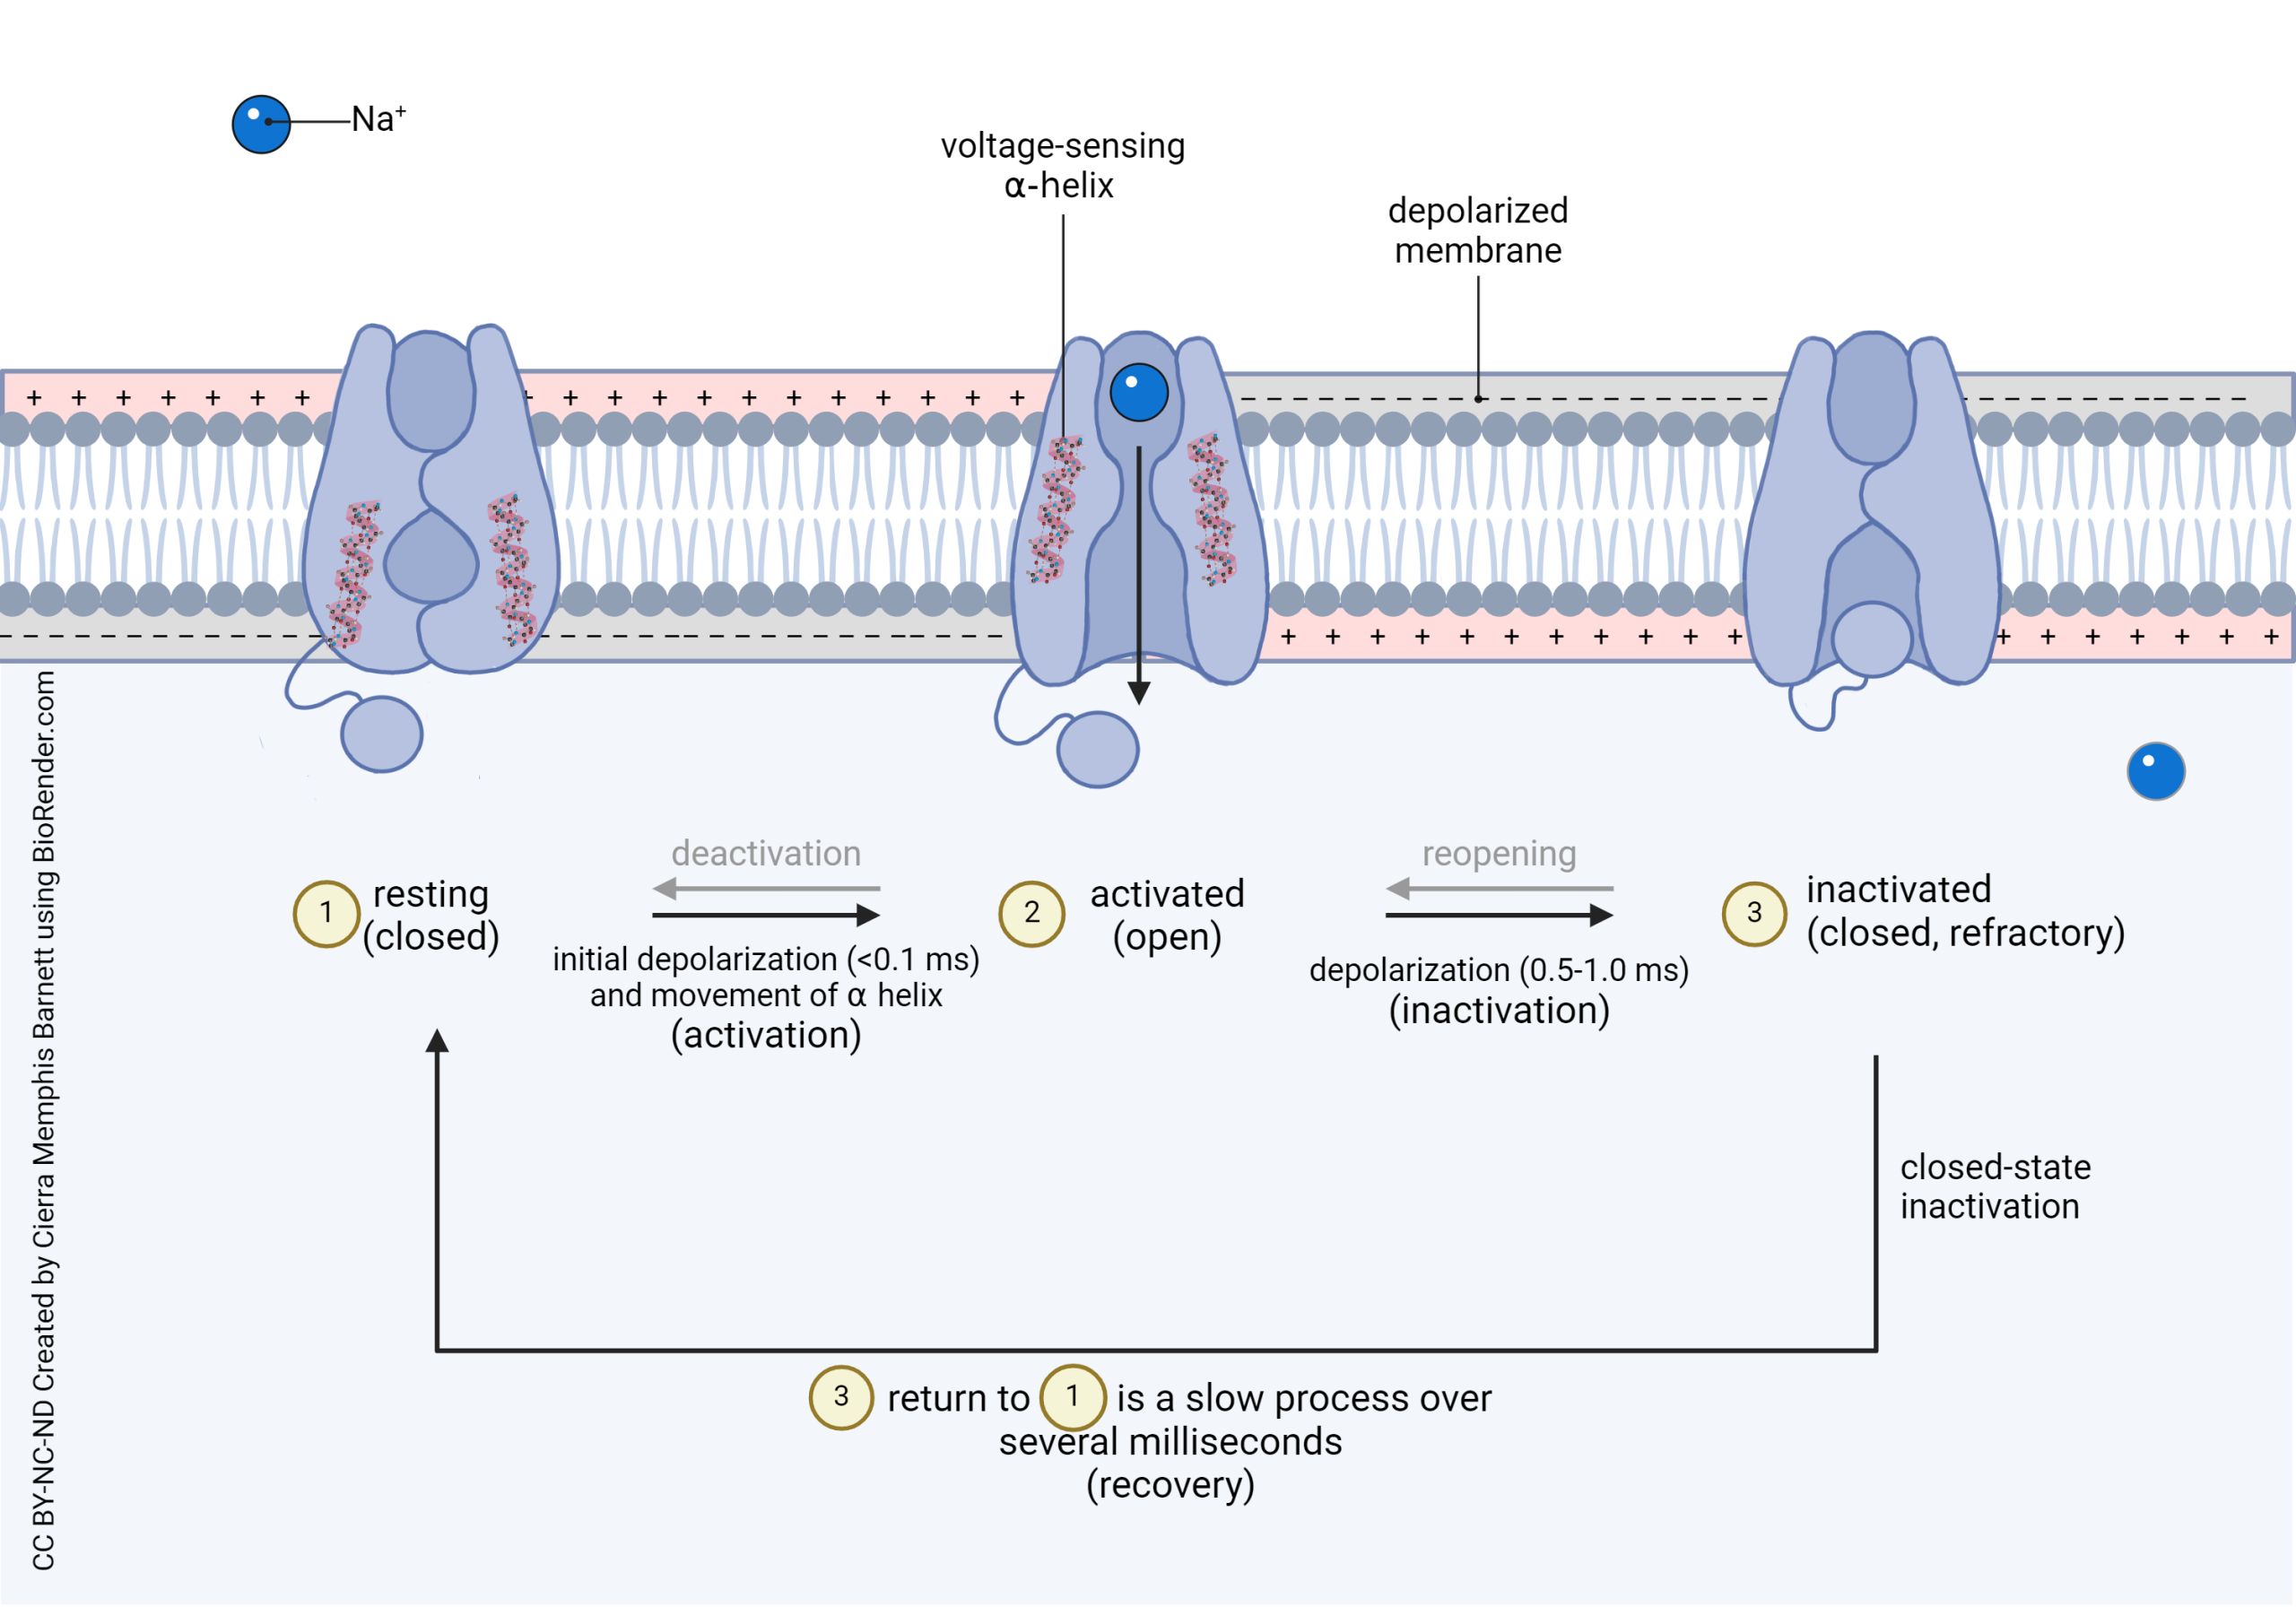
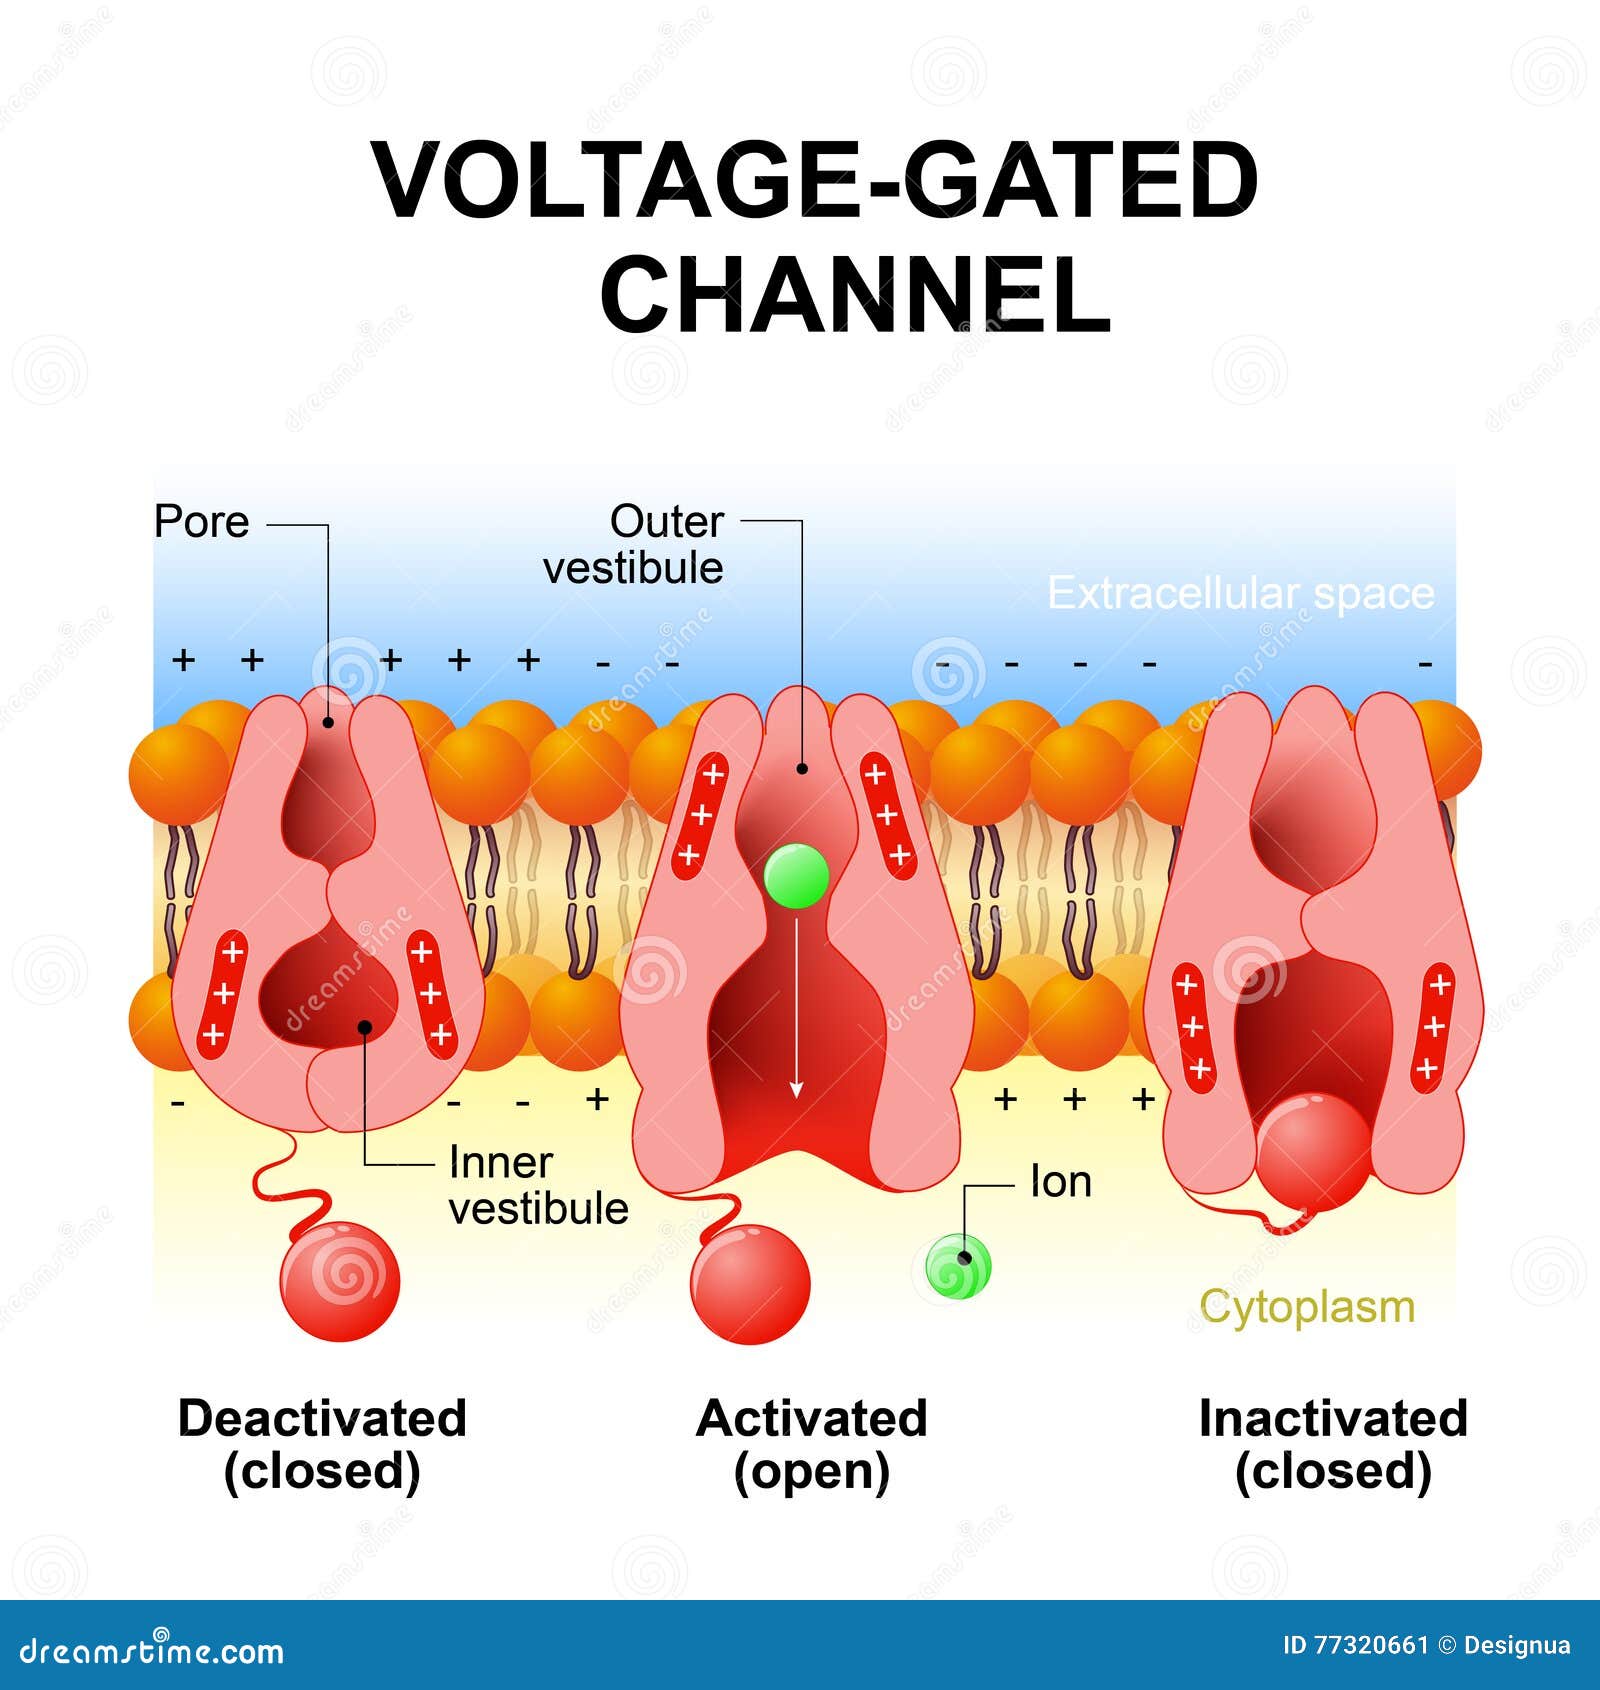
Most people learn about voltage gated ion channels from textbooks that make them sound like simple on/off switches. They're not. I spent three years patch-clamping these things in patch clamp mode, and even now I find new quirks in how they behave depending on the exact composition of my pipette solution. Let's talk about what actually happens when you work with them, not what the diagrams say. A voltage gated ion channel is a transmembrane protein complex that opens or closes its pore in response to changes in membrane potential. Sodium, potassium, calcium channels — they all share the same basic architecture. Each subunit has six transmembrane helices, labeled S1 through S6. The S4 segment acts as the voltage sensor, studded with positively charged arginine or lysine residues at every third position. When the membrane depolarizes, those charges move outward through the lipid bilayer, pulling the S4 helix and triggering a conformational change that opens the activation gate formed by the S6 helices. It sounds clean. It isn't. The actual gating current — the movement of those charges before the pore opens — is something you can measure, but only under very specific conditions. I once spent two weeks trying to isolate gating currents in a cloned hERG channel, only to realize my cells were expressing so many endogenous potassium channels that the signal was drowned out. Switched to a HEK293 line with tighter selection pressure and knocked down the background currents with 4-aminopyridine, and suddenly the gating charge displacement became visible. That kind of thing doesn't make it into the methods sections usually.
How They Actually Function in Practice
The voltage dependence of activation is described by a Boltzmann distribution. You get a G-V curve, which gives you V_half and z (the apparent gating charge). For a typical Nav channel, V_half sits around -30 to -40 mV, and z is roughly 6 to 8 elementary charges. For Cav channels, it's similar. For Kir channels — which are inward rectifiers — the voltage dependence is more complex because of internal magnesium block and polyamine sensitivity, not just gating. One thing beginners consistently miss: steady-state inactivation and activation don't have to overlap. If you're building a model and assuming the channel is only open between the activation and inactivation curves, you're probably wrong. There's often a window current where both processes are partially engaged. In Nav1.5 specifically, this window current is physiologically significant and clinically relevant — mutations that shift the inactivation curve can cause long QT syndrome or Brugada syndrome depending on the direction of the shift. I've seen grad students treat inactivation as a simple first-order process when it's actually multi-step with multiple closed inactivated states. That mismatch cost my lab about six months and a decent grant renewal because the model predictions kept diverging from the data.
Common Pitfalls When Recording From Voltage Gated Ion Channels
Series resistance compensation is the first thing to get right. If you're doing whole-cell patch clamp on a sodium channel and your series resistance is 10 megaohms, you're looking at a 10 millivolt error per nan amp of current. At peak sodium currents, which can exceed 10 nanoamps in a well-coupled cell, that's a 100 millivolt voltage error. Your command potential is wrong, your kinetics are wrong, everything is shifted. Compensate to at least 80 percent and monitor the uncompensated portion throughout the recording. If the access resistance drifts during your experiment, discard the data. It's not worth the guesswork. Another issue that comes up constantly: use-dependent block. If you're testing a drug that binds to the open or inactivated state of a sodium channel, your protocol matters enormously. A 10 millisecond pulse at -20 mV will activate far fewer channels than a 500 millisecond pulse, so the degree of block will look completely different. I've seen papers where the IC50 values differed by a factor of five simply because the test pulse duration wasn't standardized. Always report your voltage protocol explicitly. Pulse duration, holding potential, test potential, frequency of stimulation — all of it. Without that, your data is basically unusable by anyone else. There's also the problem of run-down. Calcium channels, particularly Cav1.2, tend to lose current amplitude over time in the whole-cell configuration. This isn't just a phone battery issue — it's caused by the dialysis of intracellular factors, including calmodulin and phosphorylation pathways, when you break into the cell. The solution is either to use perforated patch clamp to preserve the cytoplasm, or to include ATP and appropriate phosphatase inhibitors in your pipette solution. I routinely add 2 millimolar MgATP and 0.1 millimolar GTP, plus 10 micromolar calmodulin, and my Cav currents stay stable for at least 30 minutes. Without that, you're fitting decay curves instead of measuring real channel behavior.
Get the Full Details
Modeling Voltage Gated Ion Channels
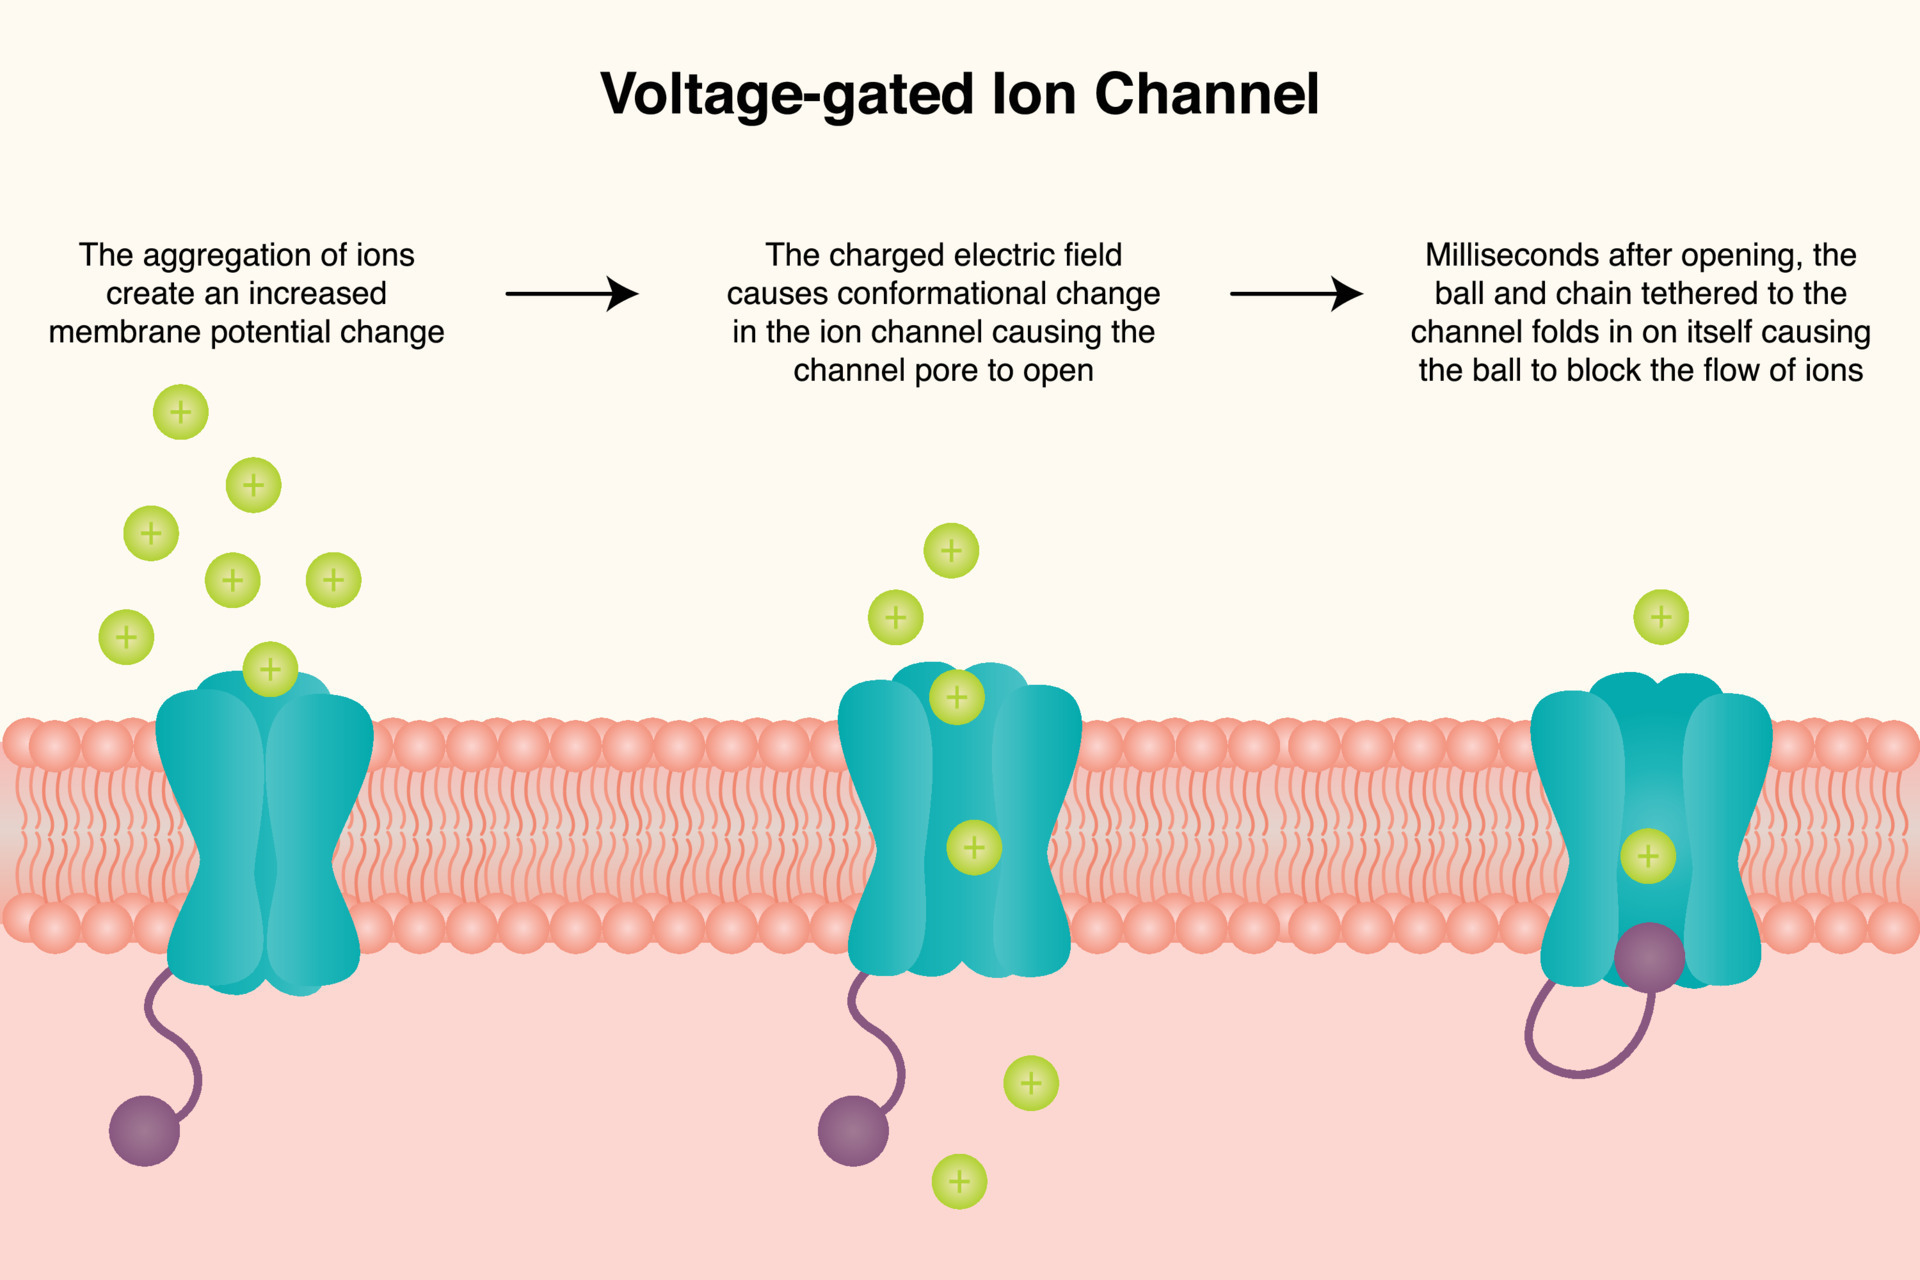
If you're building a computational model, the Hodgkin-Huxley formalism is the starting point, but it's insufficient for modern work. The original model used independent gates — m, m, m, h — which worked for the squid giant axon because the data resolution was low enough that the approximation held. Now you have single-channel recordings, cryo-EM structures, and kinetic modeling tools that can resolve individual states. Markov models are the standard. They describe each closed, open, and inactivated state explicitly, with transitions between them governed by voltage-dependent rate constants. A typical three-state Markov model for a voltage gated potassium channel has one closed state, one open state, and one inactivated state. But the real channels have multiple closed states because the S4 segments move in steps before the pore opens. A more realistic model might have four closed states, one open state, and two inactivated states. The extra states matter when you're simulating action potential repolarization — they change the recovery kinetics from inactivation, which determines refractory period. I once modeled a Nav channel with only two closed states and got action potential shapes that looked reasonable until I tried to reproduce the effect of a fast versus slow heart rate on APD90. The rate dependence was completely wrong because the recovery from inactivation didn't track the experimental data at higher frequencies.
Pharmacology and Voltage Gated Ion Channels
The drug discovery space around these channels is massive. Cardiac sodium channel blockers, calcium channel blockers for hypertension, potassium channel openers for asthma — they all target voltage gated ion channels. The challenge is selectivity. Many compounds that look selective in a heterologous expression system turn out to hit multiple channel subtypes at therapeutic concentrations. A compound you think is blocking Nav1.7 for pain modulation might also be blocking Nav1.5 in the heart at a 10-fold lower concentration. Always do a screening panel across the major isoforms. Nav1.4 skeletal, Nav1.5 cardiac, Nav1.7 sensory, Cav1.2, Kv1.5 atrial, KCNQ1 — that's the minimum panel I run before considering any compound further along. There's also the issue of state-dependent binding that I mentioned earlier, but it deserves emphasis. Many channel blockers preferentially bind to the inactivated state. That means the potency you measure depends on how much time the channel spends in that state, which depends on your protocol. A drug that looks like a potent blocker at 0.1 hertz might look nearly inactive at 1 hertz because the channels don't have time to inactivate between pulses. Or vice versa — if the drug stabilizes the inactivated state, increased frequency could enhance block. This is called use-dependent or frequency-dependent block, and it's why antiarrhythmic drugs like flecainide show what's called the Class I C subdivision in the Vaughan Williams classification. They block sodium channels with slow unbinding kinetics, so they accumulate with each beat during tachycardia.
Where the Field Stands Now
Cryo-EM has transformed structural understanding of voltage gated ion channels. We now have high-resolution structures for NavAb, NavRh1, Kv1.2, CavAb, and several mammalian channels. These structures have revealed details about the voltage sensor domain that electrophysiology alone couldn't resolve — the precise tilt of S4, the water-filled crevices that allow charged residues to interact with the extracellular medium, the lipid molecules that sit in the interface between the voltage sensor and the pore domain. But structure doesn't equal function. A static snapshot tells you where things are, not how they move. Combining cryo-EM with molecular dynamics simulations and electrophysiology gives you the most complete picture, but each technique has blind spots. The biggest open question right now is how auxiliary subunits modulate channel behavior. Beta subunits for sodium channels, beta subunits for calcium channels, KCNE proteins for potassium channels — they're all crucial for proper trafficking, kinetics, and pharmacology, but their mechanisms aren't fully understood. In my own work, adding the beta-1a subunit to Nav1.7 shifted the voltage dependence of activation by 8 millivolts in the hyperpolarized direction and accelerated inactivation by roughly 30 percent. Those aren't trivial changes. They mean the channel opens more easily and shuts faster, which has real consequences for neuronal excitability. Any study that expresses a voltage gated ion channel without its native auxiliary subunits is working with a simplified version that may not reflect physiology. If you want to dig deeper, the IUPHAR/BPS Guide to Pharmacology has detailed entries on every cloned voltage gated ion channel with references to the key papers. ChannelsAndDrugs.com is another useful resource. For hands-on patch clamp work, the Axon Manual of Patch Clamp Applications is still the most practical guide available, even though it's been out for a while. The fundamentals haven't changed much, and the troubleshooting sections are worth more than most of the newer textbooks.