The Real Drivers of Population Density
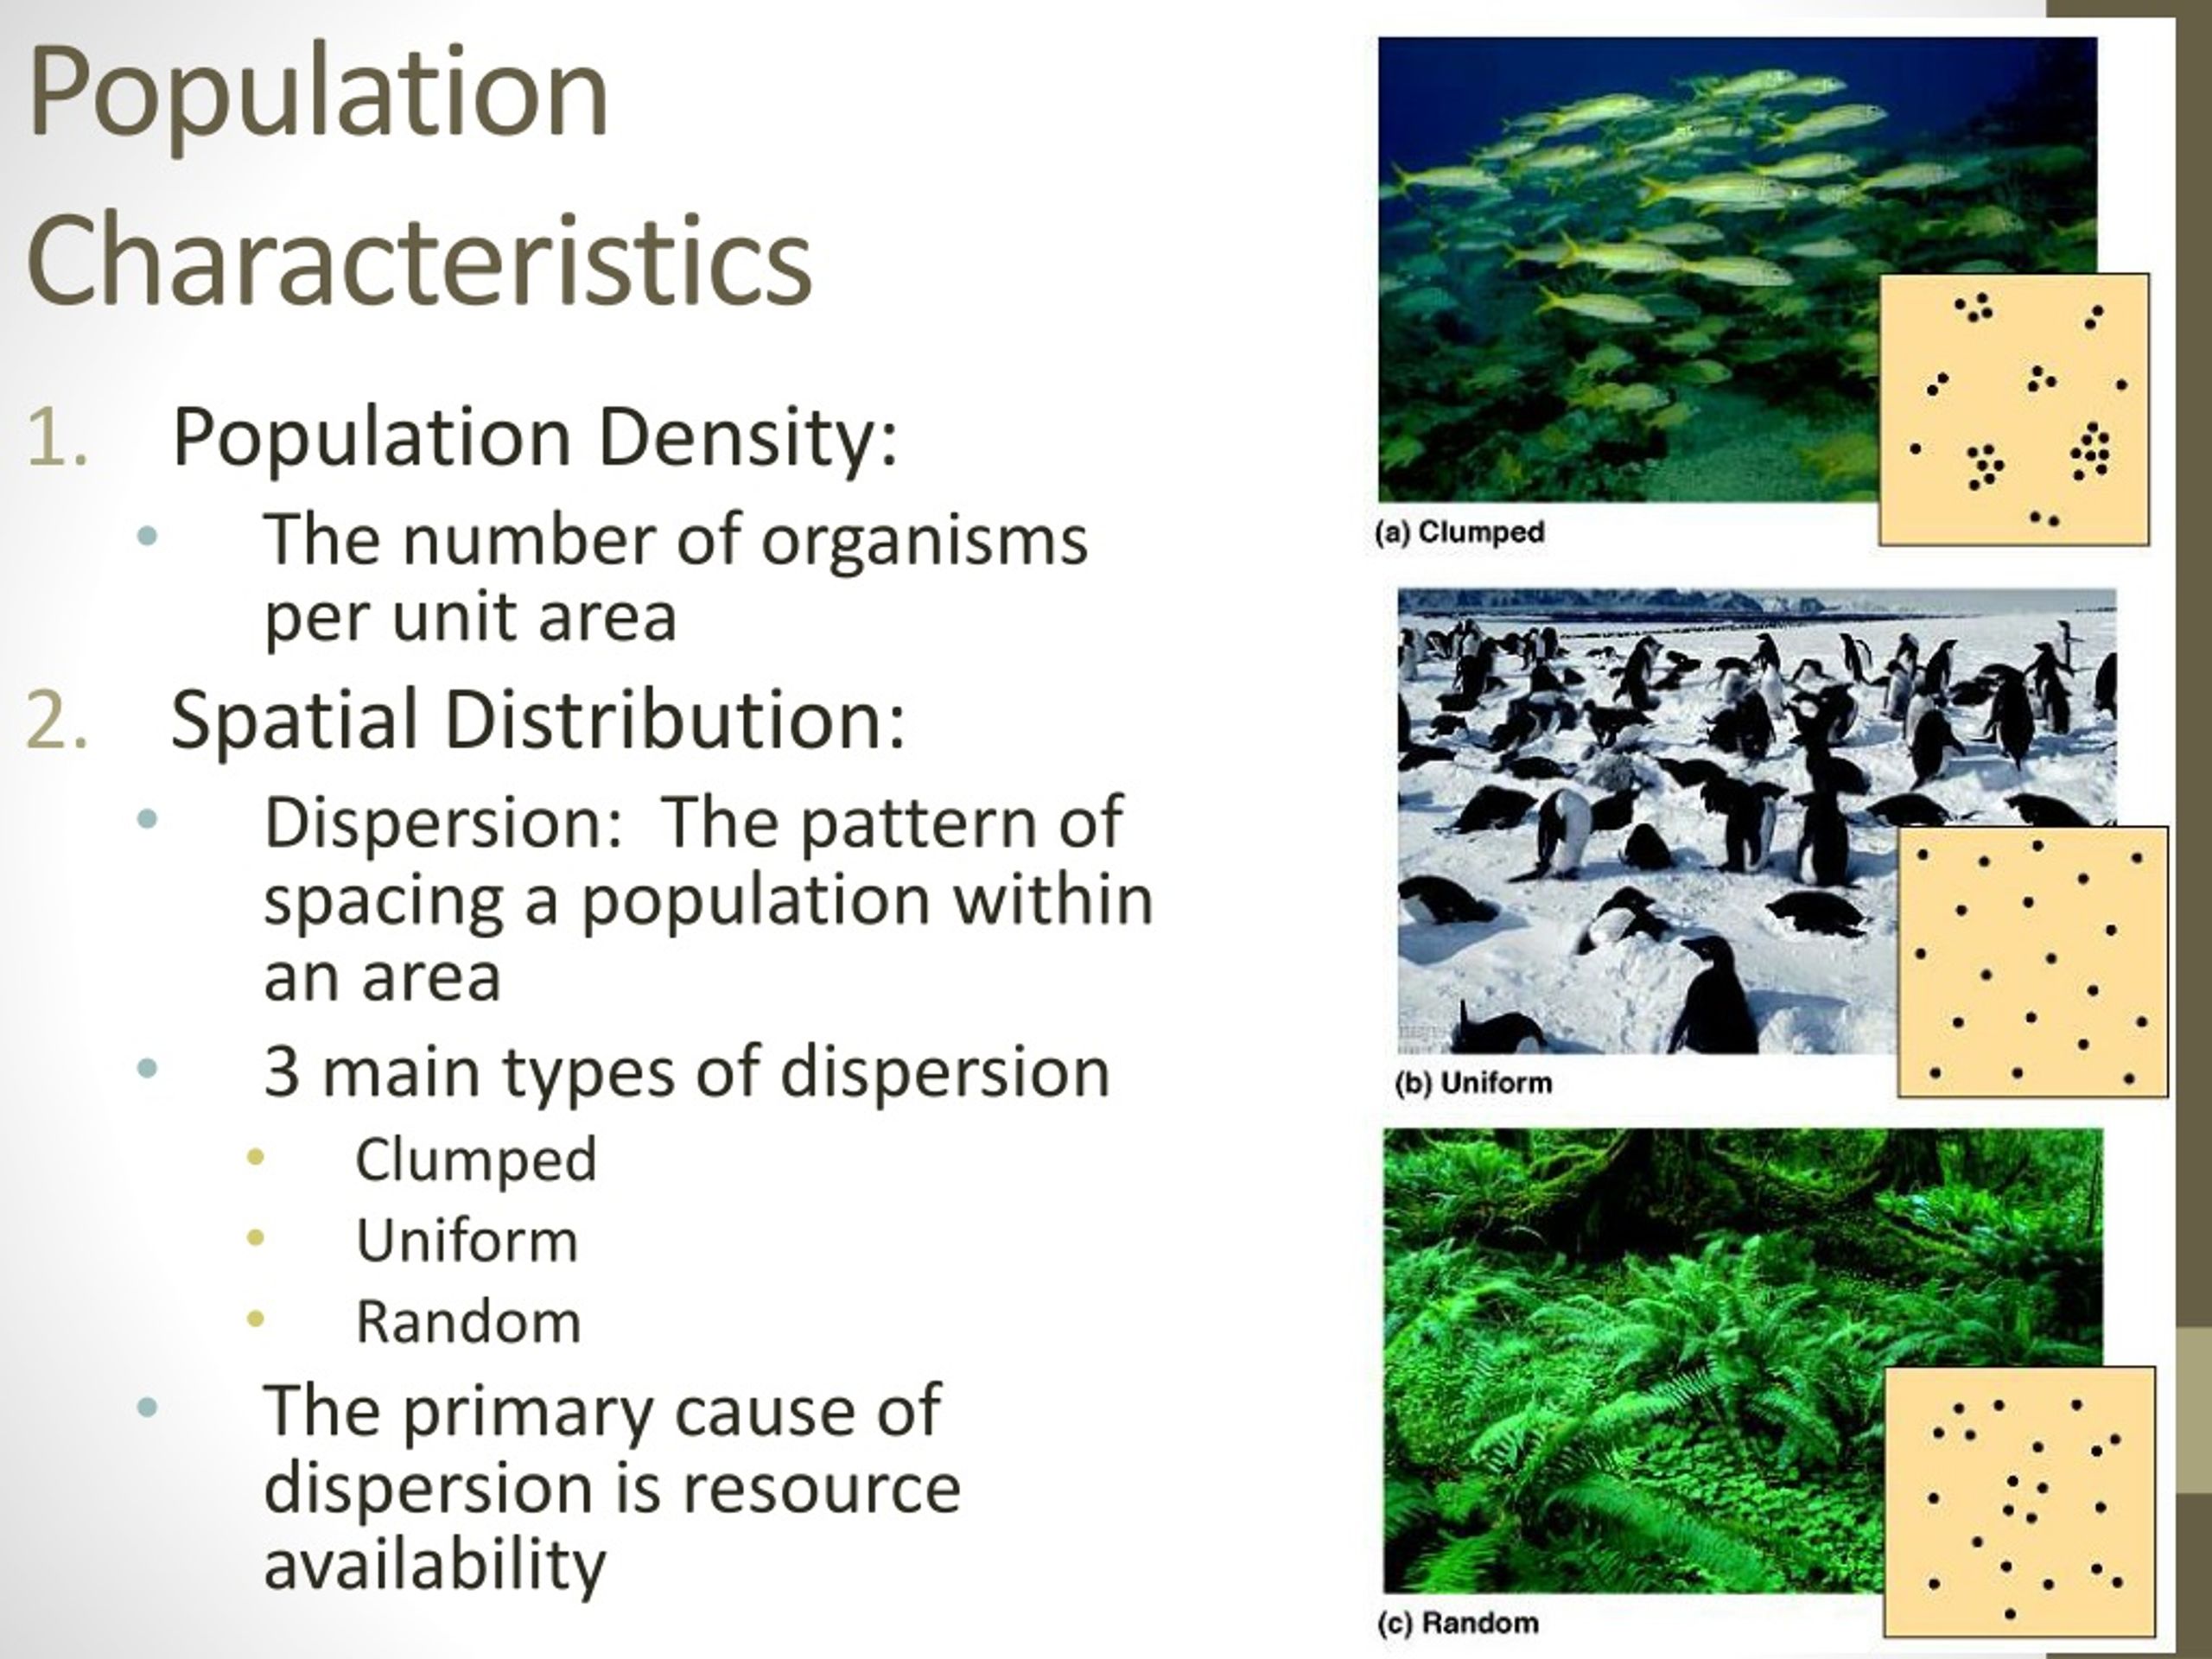
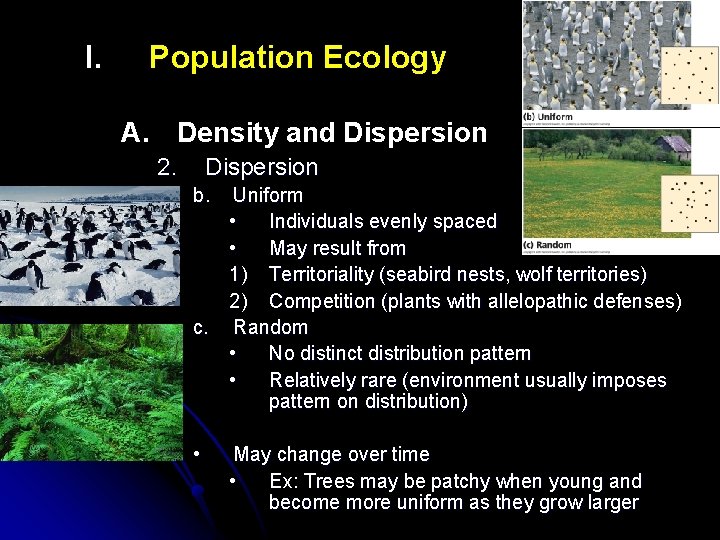
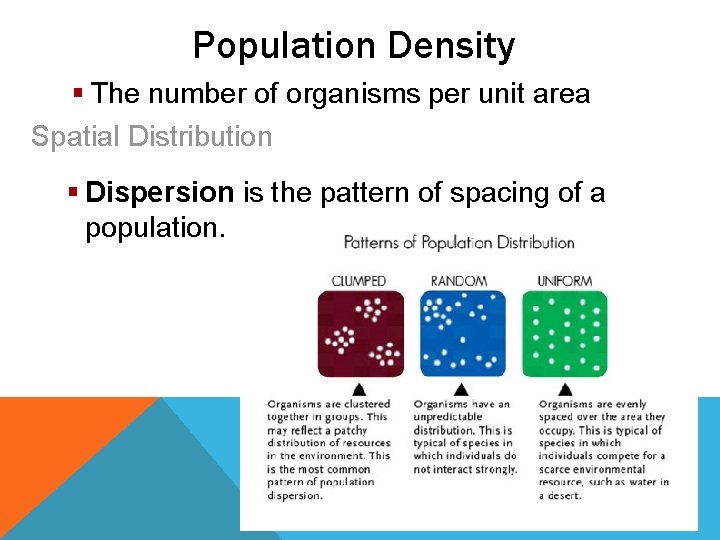
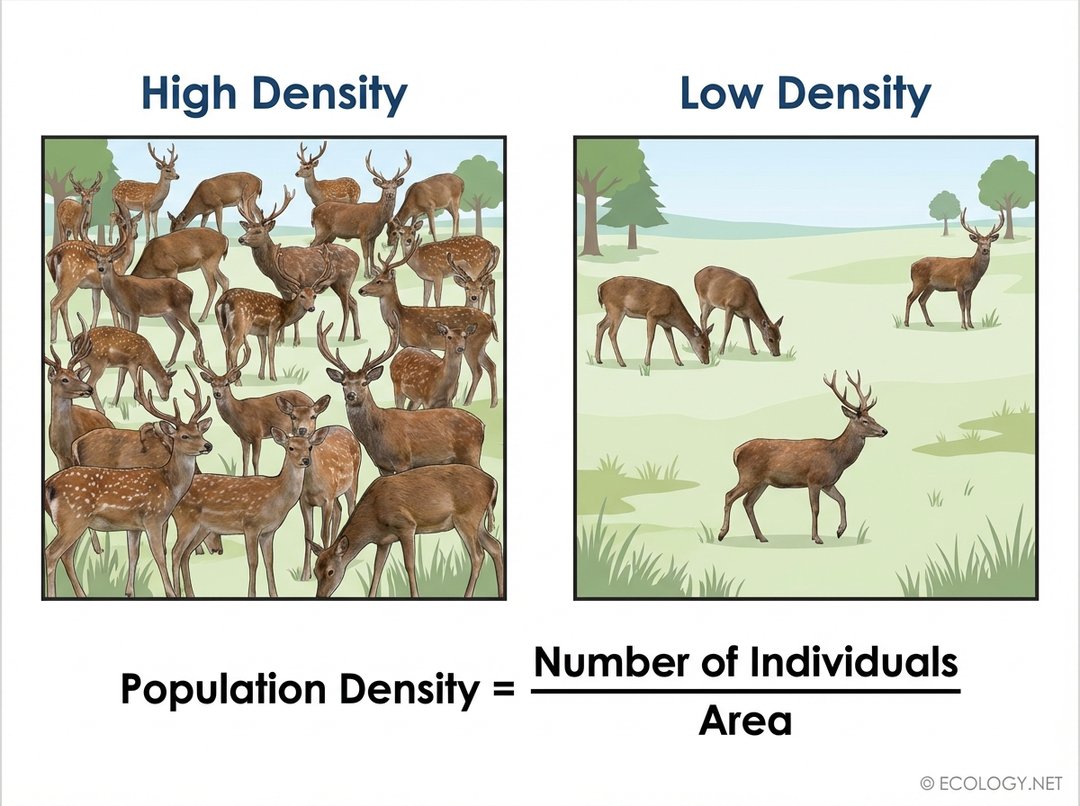
Population density is just a ratio of individuals per unit area or volume. That's it on the surface. But the factors that actually shift that number are messy, interconnected, and frequently misunderstood by anyone who learned this from a textbook diagram alone. The four big categories are always birth rate, death rate, immigration, and emigration. These are the demographic accounting terms. If births plus immigrants exceed deaths plus emigrants, density rises. If the opposite happens, it falls. That's not where the real work begins though. The real question is what controls each of those four variables in any given environment. Biotic factors come first in practice. Resource availability is the obvious one, but most people gloss over how resource distribution pattern matters more than total resource quantity. A patchy distribution of food can keep density locally high in certain microhabitats while the broader area looks sparse on paper. Predation pressure does the same thing, often creating density refugia where prey clusters around defensive features. Competition, both intra- and inter-specific, can suppress density well below what resources alone would suggest. Disease transmission rates scale with density in most cases, creating a natural brake that kicks in harder the more crowded things get.
Abiotic factors set the ceiling. Temperature, moisture, salinity, pH, and light availability all determine the fundamental niche. A population might be perfectly capable of reaching higher density if temperature were five degrees warmer, but the abiotic constraint keeps it where it is. Seasonal fluctuations in these factors cause corresponding density swings that annual snapshots completely miss. I once spent three weeks trying to figure out why a deer population appeared to crash in autumn survey data when in reality it was just a seasonal displacement into adjacent cover types. The animals hadn't died or left the landscape. They had moved vertically and horizontally within it, and my trap lines missed them entirely. Land availability and habitat structure matter enormously and are frequently conflated. A forest fragment might hold the same carrying capacity for a bird species as a larger contiguous forest, but only because edge effects have already degraded the interior quality. Density calculations that ignore habitat heterogeneity will systematically overestimate viable population sizes in fragmented landscapes. Human disturbance operates as both a biotic and abiotic force depending on context. Noise pollution, artificial lighting, fragmentation, and direct persecution all compress effective density by reducing usable habitat area without changing the total geographic area. This is why density estimates from protected areas often fail to translate to unprotected surrounding landscapes.
There is one counter-intuitive point that catches people out repeatedly. Higher resource availability does not always produce higher density. In some systems, increased resources trigger dispersal behavior rather than aggregation. A classic example involves certain fish species in nutrient-rich lakes where individuals spread out to maximize individual foraging efficiency instead of clustering. The population density per square kilometer can actually decrease when you enrich the system. This is the so-called ideal free distribution in action, and it means your intuition about "more resources equals more crowding" is wrong more often than you'd expect. Another nuance is density-dependent versus density-independent mortality. Students learn the difference but rarely internalize that both operate simultaneously. A harsh winter kills a fixed proportion of a population regardless of how dense it is. But the survivors face a slightly different competitive landscape that changes their reproduction rate going forward. These two forces layer on top of each other every single year, and disentangling their contributions from observational data is extraordinarily difficult. You need multi-year time series with proper control sites, not a single census. I ran into this problem head-on working with a small mammal study where we had annual trapping data across twelve sites. The population at one site showed a dramatic density decline that correlated perfectly with a cold snap the following winter. The easy conclusion was that cold weather caused the crash. But when I looked at the predator scats from the same sites, we found a threefold increase in predation marks during the years following any density peak, regardless of weather. The real pattern was a delayed density-dependent response through predator numerical reaction, not an immediate weather effect. The weather variable was a confounder that looked important because we weren't tracking the predator population simultaneously. That cost us about six months and a considerable amount of patience before we redesigned the monitoring protocol to include predator indices at every site.
Get the Full Details
The methodological side deserves attention because density estimates are only as good as the method used to derive them. Mark-recapture gives you density only if you can define the population boundary accurately, which is nearly impossible for mobile species over large areas. Quadrant sampling works for plants and sessile organisms but introduces huge edge effects near boundaries. Distance sampling assumes perfect detection at the transect line, which is never true, and the correction factors add uncertainty that many papers quietly bury in supplementary material. Each method has a different detection probability curve, and comparing density estimates across studies that used different methods is essentially meaningless without conversion factors that rarely exist. Scale is another trap. Density measured at a quarter-hectare plot might tell you nothing about density at a forty-hectare landscape. Organisms respond to environmental gradients at different scales, and the grain of your sampling determines what pattern you see. This is why meta-analyses of population density across species often produce noise rather than signal, because the studies weren't sampling at comparable scales. There's also the issue of temporary versus permanent residents inflating density counts. Migrants passing through an area will register in a snapshot census but contribute nothing to the reproductive dynamics of the local population. For birds especially, breeding density and total density can differ by orders of magnitude depending on the season of your survey. I've seen reports where the "population density" of a wetland was based entirely on wintering waterfowl counts that included thousands of transient individuals moving through on migration, making the site appear far more important as habitat than it actually is for resident species.
The mathematical models that predict density changes assume constant parameters, which is another way of saying they almost never hold up in real ecosystems. Ricker and Beverton-Holt models work fine for fisheries with heavily monitored stocks. They fall apart quickly for anything with irregular breeding intervals, age-structured populations with overlapping generations, or environments where the carrying capacity itself fluctuates year to year. Using a static K value for a species in a drought-prone region is just storytelling with numbers. Ultimately, population density in ecology is not a single-number fact you can record and file away. It is a snapshot of a dynamic equilibrium between opposing forces that shift at different rates and on different scales. The factors that matter change depending on whether you are looking at a bacterium in a petri dish or a wolf pack across a hundred thousand hectares. The trick is knowing which scale and which mechanism dominates in the system you are studying, and being honest about the uncertainty when you report the number.