Monosaccharides and Why They Matter in Practice
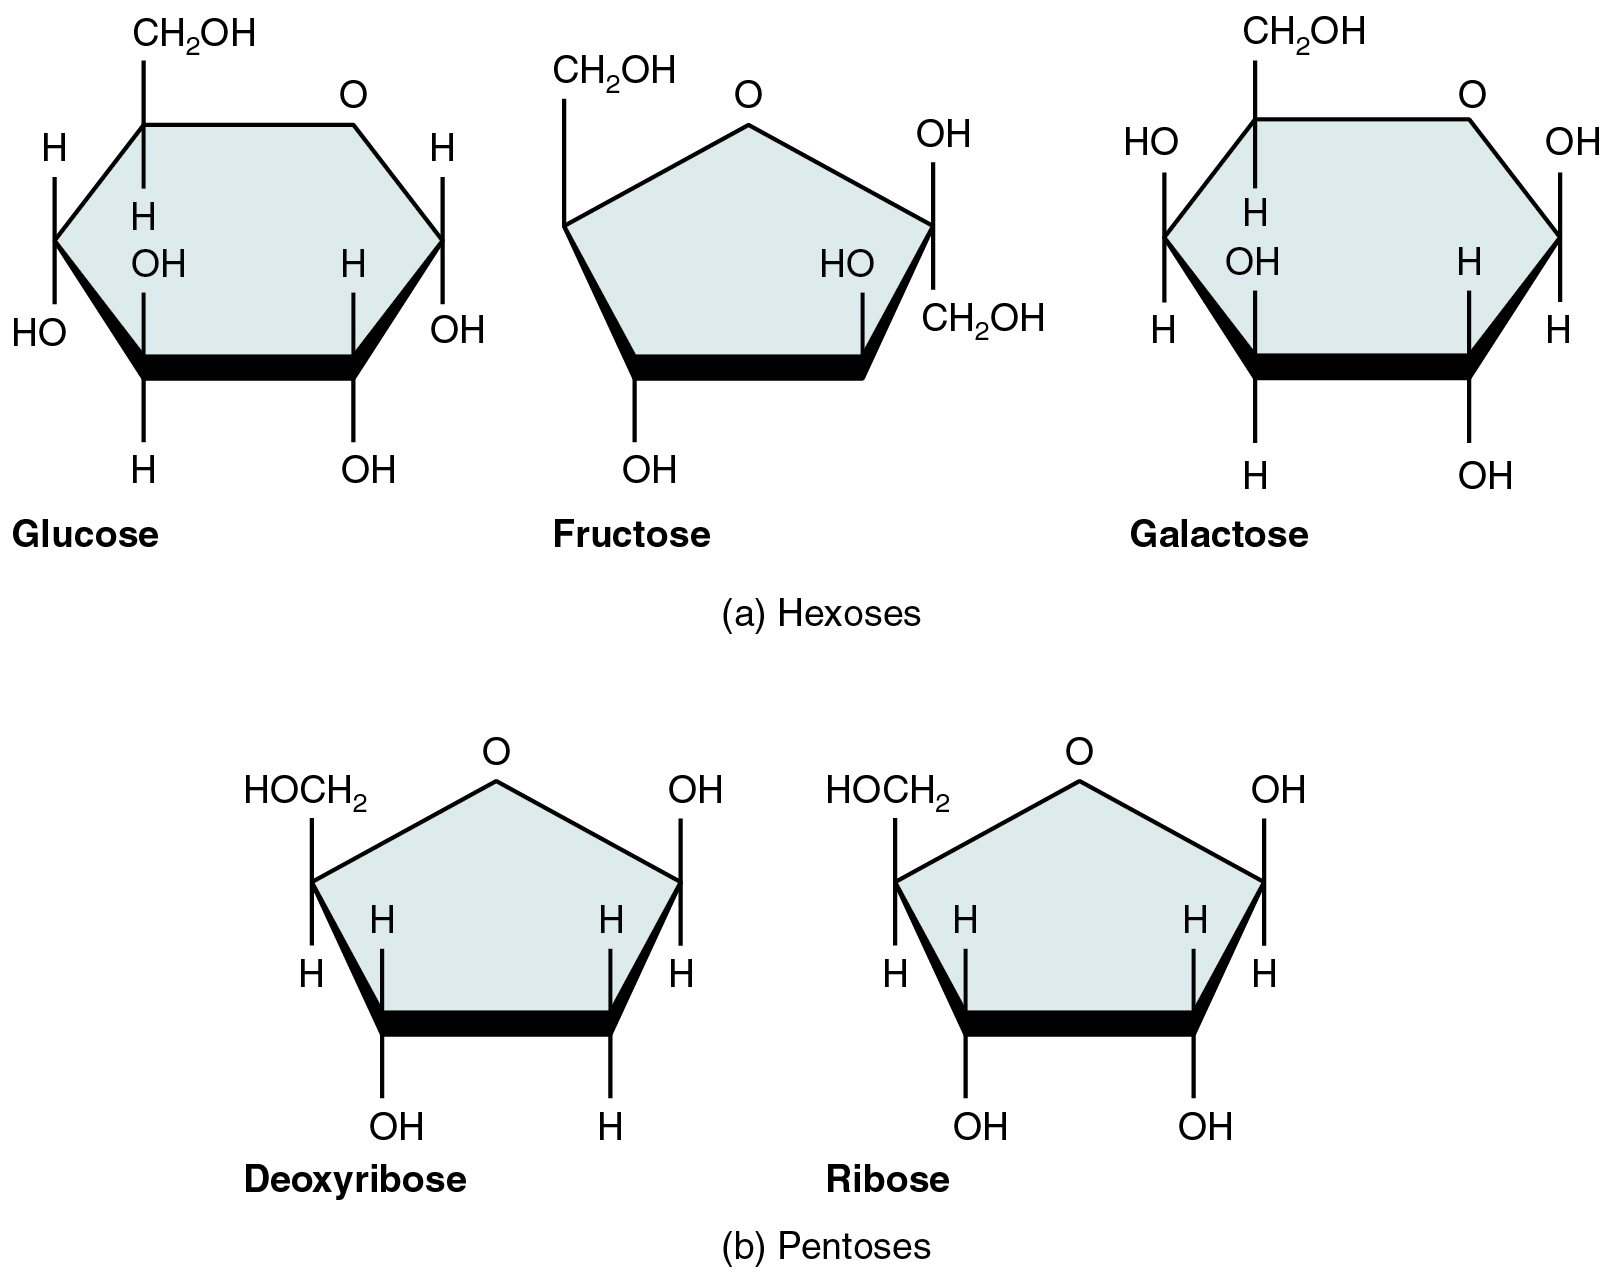
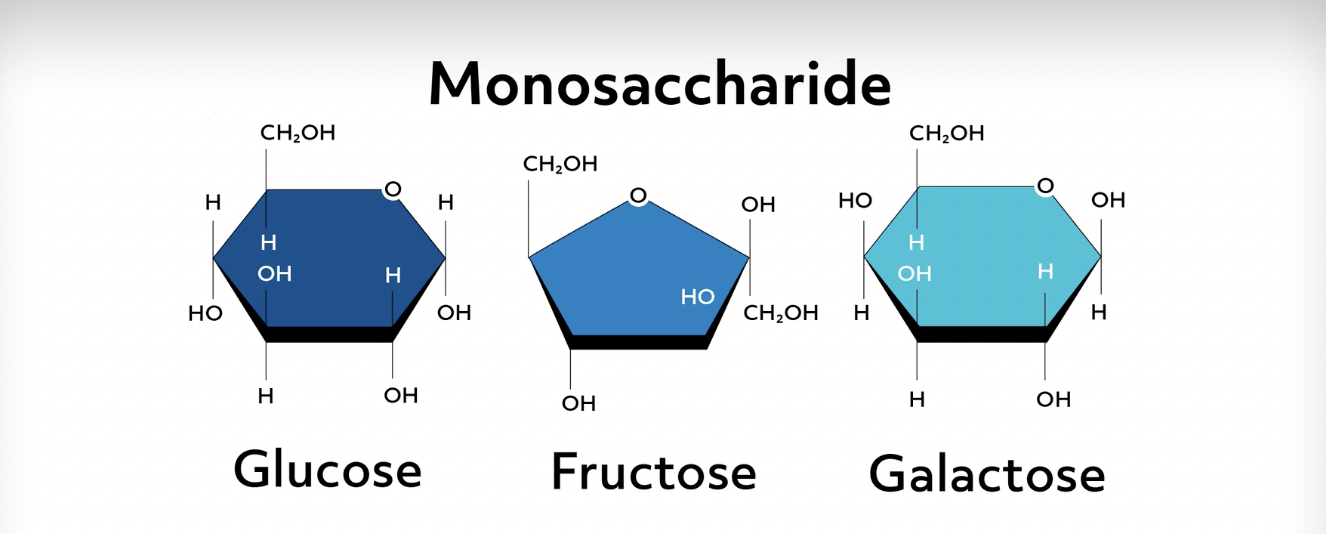
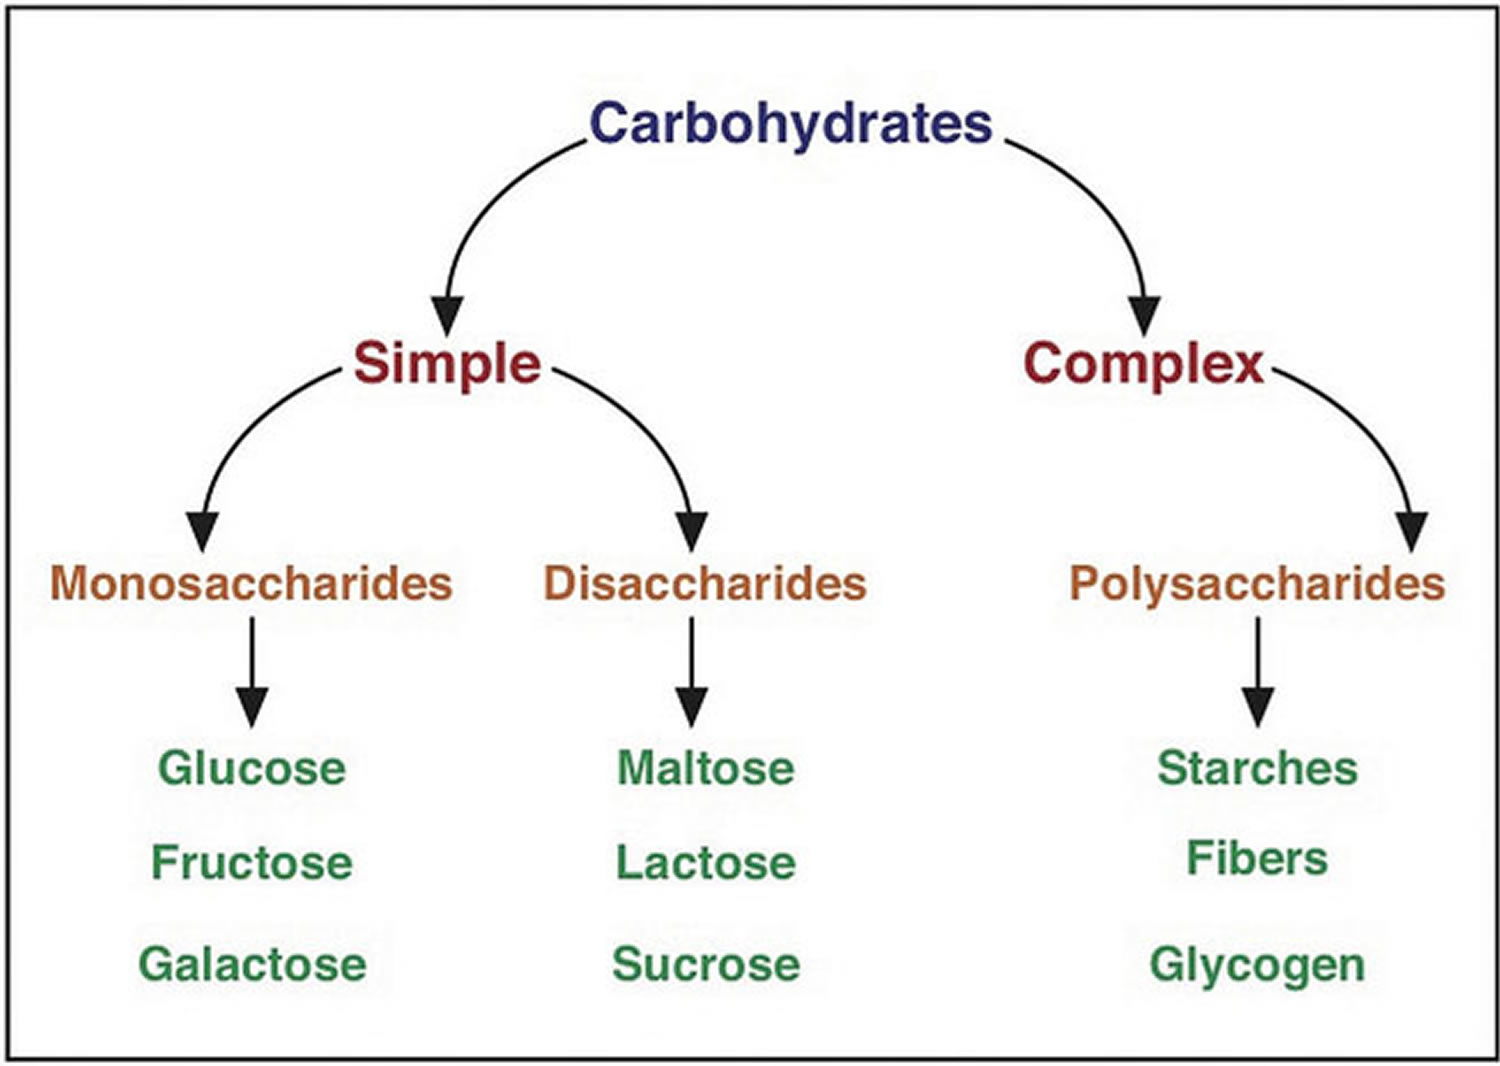
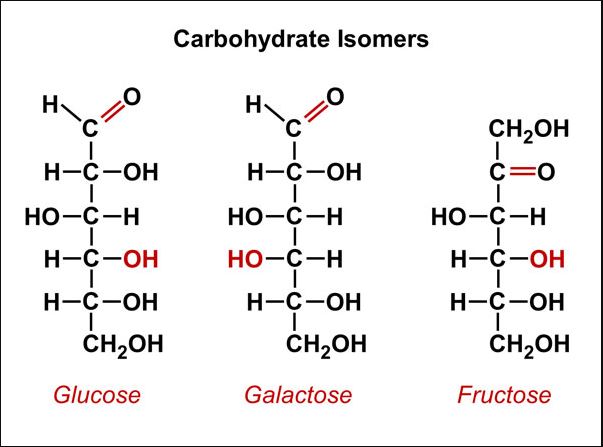
Carbohydrate monomers are the single sugar units that stitch together to form complex carbohydrates. The most basic form is a monosaccharide — molecules like glucose, fructose, and galactose, each carrying the general formula Cn(H2O)n. You can think of them as individual LEGO bricks. By themselves they do certain things. When linked by glycosidic bonds, they become disaccharides, oligosaccharides, and polysaccharides. The standard examples you see in every textbook are glucose, fructose, and galactose. They all share C6H12O6 but differ in how their atoms are arranged. That structural difference is what makes glucose an energy substrate your cells actually use directly, while fructose has to be processed through the liver first. Galactose doesn't really show up alone in food — it comes attached to glucose in lactose. Understanding these distinctions matters when you're looking at anything from metabolic pathways to food labeling.
What Are Carbohydrate Monomers
At their core, carbohydrate monomers are single sugar units that serve as the building blocks for larger carbohydrates. The primary types include hexoses like glucose and fructose, pentoses like ribose and deoxyribose, and smaller three-carbon sugars like glyceraldehyde. Each one acts independently, but their real functional value appears when they polymerize into starch, cellulose, glycogen, or other complex chains. The glycosidic bond is the key structural feature here. When two monosaccharides join, an oxygen bridge forms between them through a condensation reaction that releases a water molecule. The configuration of that bond — alpha or beta — determines everything about the resulting polymer. Alpha-1,4 linkages create helical structures like starch. Beta-1,4 linkages create straight, rigid chains like cellulose. Same monomer, completely different physical properties. That's not theoretical. It affects how things digest, how they're stored, and how they break down industrially. I ran into this exact problem a while back working on an enzyme hydrolysis optimization project. We were trying to selectively break down starch without touching the cellulose present in the same feedstock. Standard amylose-targeting enzymes started nibbling at the cellulose too, probably because industrial-grade starch always has some microcrystalline contamination. The workaround was switching to a two-step process where we pre-treated with a cellulase inhibitor at controlled pH before introducing the amylase. It added about 40 minutes to the protocol but cleaned up the product spectrum significantly. You don't learn that from a diagram.
The Structural Details That People Skip
Ring formation is something beginners usually gloss over. In solution, monosaccharides don't stay in their straight-chain form. Glucose cyclizes into either a six-membered pyranose ring or a five-membered furanose ring. The equilibrium in water at room temperature sits at roughly 64% beta-pyranose, 36% alpha-pyranose, and trace amounts of the other forms. Fructose does something similar but skews much heavier toward furanose. This isn't academic — ring conformation dictates how enzymes recognize and bind these molecules. Maltose and cellobiose are both made from two glucose units, but the beta linkage in cellobiose makes it completely invisible to the same amylase that chews through maltose. Specificity comes from that one bond orientation. Mutarsation is another thing worth understanding practically. When you dissolve crystalline alpha-D-glucose in water, the optical rotation of the solution changes over time until it stabilizes. That's the alpha form converting to the beta form through the open-chain intermediate until they reach equilibrium. It happens within hours at room temperature. If you're doing any kind of analytical work — refractometry, polarimetry, enzymatic assays — you need to account for this. Running a measurement on freshly dissolved crystals gives you a different reading than the same solution sitting for a day. Standardize your dissolution protocol or your data becomes noise. Common pitfall: people assume all simple sugars behave identically in reactions because they share the same molecular formula. They don't. Glucose and fructose react differently with Benedict's reagent, ferment at different rates through yeast, and have entirely different metabolic routing once absorbed. Treating them as interchangeable in formulation or experimental design will cost you time and bad results.
Get the Full Details

Polymerization and Real-World Implications
When monomers link up, the directionality of the chain matters. Each glucose unit in a polysaccharide has a reducing end and a non-reducing end. Enzymes read those ends differently. Glycogen synthase adds glucose to the non-reducing end. That's why glycogen branching happens the way it does — it creates lots of exposed non-reducing ends for rapid mobilization when your body needs quick glucose release. Starch works similarly but with far fewer branches. Cellulose has no branches at all, which is why it packs into fibers instead of compact granules. The practical implication shows up in food science and biofuel production. Breaking down cellulose into fermentable sugars requires either strong acid treatment or specialized cellulase cocktails, and neither approach is cheap at scale. That's the main bottleneck in second-generation bioethanol. Meanwhile, breaking down starch is straightforward and economical, which is why first-generation biofuel from corn or sugarcane works fine but raises the food-versus-fuel question. The monomer itself is the same glucose either way. The bond type is what creates the entire economic and logistical difference. Limitation to keep in mind: monosaccharide analysis by standard HPLC can struggle with co-elution. Glucose, fructose, and sucrose often overlap on basic C18 columns. You need either a specialized amino-bonded column or ion-exchange chromatography with pulsed amperometric detection to get clean separation. If you're getting messy peaks and assuming they're pure compounds, you're probably wrong. Running a standard mix alongside your sample cuts that confusion down to something manageable in about 20 minutes.
Iodine testing is still useful for identifying starch presence even though it's old-school. The helical amylose structure traps iodine molecules and turns deep blue. It won't tell you anything about monosaccharides directly, but it's a quick way to check whether your hydrolysis reaction actually worked. If the blue color disappears after treating a starch suspension with amylase, your enzyme is active. Takes thirty seconds and costs almost nothing compared to running a full assay. The take-it-or-leave-it part is this: knowing what carbohydrate monomers are structurally tells you very little about how they behave in real systems. The bond geometry, the ring conformation, and the biological context around each sugar determine everything that actually matters in practice. Textbooks cover the first part. The rest comes from doing the work and watching what breaks.