Evolution doesn't happen in a vacuum. Something is always pushing on a population.
I ran into this the hard way when I was designing a bacteriophage resistance experiment with E. coli back in grad school. I had plates of bacteria growing under what I thought were identical conditions, and one batch evolved resistance while the other didn't. It turned out the incubator on one side of the lab had a slightly higher airflow velocity, which changed the evaporation rate on the agar surface. That tiny difference in water activity became a selective pressure that shifted the whole trajectory of the culture. The lesson was that selective pressures don't have to be dramatic or intentional. They just have to exist and they will act on variation whether you notice them or not. Selective pressures are any external factor that affects the survival or reproductive success of individuals within a population. They come from biotic sources like predators, parasites, competitors, and available mates, or abiotic sources like temperature, salinity, pH, radiation, and resource availability. When a selective pressure is present, individuals with certain heritable traits reproduce more successfully than others. Over generations, this changes allele frequencies in the population. That change is natural selection in action. The mechanism itself is straightforward but the practical implications are often misunderstood. Here is how it actually works when you are dealing with real organisms rather than textbook examples.
You start with genetic variation in a population. This variation can come from mutation, recombination, gene flow, or horizontal gene transfer depending on the organism. Not all variation matters equally. Only the heritable portion is relevant for evolution. Phenotypic plasticity can confuse the picture because it produces variation in traits without changing allele frequencies, but plasticity itself can evolve if the environment makes flexibility advantageous. A selective pressure acts on that variation by making some phenotypes more likely to survive and reproduce than others. The pressure doesn't create the variation. It filters it. This distinction matters because people often describe selection as if it were directing evolution toward a goal. It isn't. Selection is a sieve, not an architect. The strength of a selective pressure determines how fast evolution proceeds. Strength is measured as the selection coefficient, usually denoted as s. If a genotype has a fitness of 1.0 and another has a fitness of 0.9, the selection coefficient against the weaker genotype is 0.1. In bacteria with generation times measured in minutes, even small selection coefficients produce measurable change within hours. In large, long-lived mammals, the same coefficient would take decades or centuries to shift allele frequencies noticeably. Time scale and population size interact with selection strength in ways that are easy to miss if you are only thinking in one direction.
Types of selection and what they actually look like
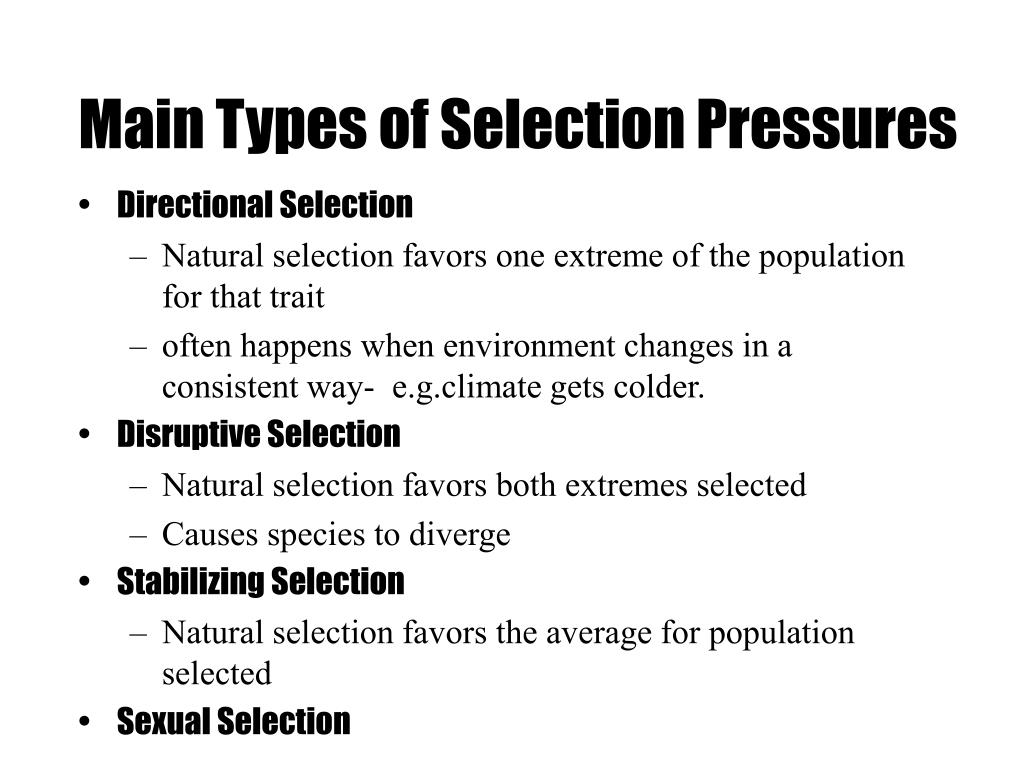
Directional selection shifts a trait mean in one direction. This is the classic example most people picture. A population of beetles where darker individuals survive better on dark soil because birds can see them less easily. Over generations the population gets darker. But directional selection is not always clean. In natural populations you often see a mix of opposing pressures that partially cancel each other out. A trait that improves mating success might simultaneously reduce survival. The observed mean sits somewhere between what each pressure alone would produce. Stabilizing selection reduces variance around an optimum. Human birth weight is the textbook case. Babies that are too small have poor survival. Babies that are too large face complications during delivery. The optimal range sits in the middle and individuals at the extremes are selected against. This type of selection is often underappreciated because it doesn't produce obvious change. It maintains the status quo by weeding out deviations. In a lab setting, stabilizing selection is what keeps inbred lines relatively stable across generations as long as you don't change the environment. Disruptive selection favors extremes over intermediates. This is rarer in nature but it matters because it can be a precursor to speciation. If two different ecological niches exist within a habitat and the intermediates cannot exploit either effectively, you can get a bimodal distribution forming. I saw a version of this in a fish population study where a lake had both open water and dense vegetation zones. Intermediate-sized fish were inefficient in both habitats and their fitness dropped relative to the specialists at each end. The population was on its way to diverging, but it took multiple generations and a lot of gene flow was still happening, so the split never fully completed before the study ended.
Get the Full Details

Common pitfalls that trip people up
The biggest mistake I see is assuming that every trait exists because of selection. Some traits are byproducts of other selected features. The red color of male peacocks is linked to overall health and parasite resistance, not selected for color itself. Correlated traits complicate everything. When you select for one thing, you get other things along for the ride. This is why artificial selection programs sometimes produce unexpected side effects. Another issue is ignoring the timescale. Selective pressures operate continuously, but evolution is often thought of as something that happens in big visible jumps. Most of the time allele frequency changes are subtle and cumulative. You need controlled comparisons over many generations to detect them reliably. Without replication and proper controls, you are just observing noise and calling it evolution. Sexual selection is a subset of selective pressure that people frequently conflate with natural selection. It operates through mate choice and competition for mates rather than survival per se. A trait can be selected for even if it reduces survival, as long as the reproductive advantage outweighs the mortality cost. The handicap principle describes this dynamic, though the empirical support for it is mixed depending on the species and trait in question.
Frequency-dependent selection is another nuance that doesn't get enough attention. In negative frequency-dependent selection, rare phenotypes have an advantage. Predator search images are a common mechanism. Predators learn to recognize the most common prey form, which gives rare morphs a temporary survival edge. As rare morphs become common, the advantage flips. This can maintain polymorphism in populations without requiring any heterozygote advantage at the genetic level.
Measuring selective pressures in practice
If you want to study selective pressures rather than just talk about them, you need quantitative data. The standard approach involves estimating fitness differences between genotypes or phenotypes. You can do this through mark-recapture studies, pedigree analysis, or controlled laboratory experiments. The key is that you need to measure actual reproductive output, not just survival. An organism that survives but doesn't reproduce contributes nothing to the next generation. The breeder's equation, R = h²S, is the workhorse for predicting response to selection. R is the response, h² is heritability, and S is the selection differential. It sounds simple but applying it correctly requires accurate estimates of heritability, which in turn requires controlled breeding designs or genomic relatedness matrices. Genomic tools have made this much more feasible than they used to be, but the assumptions still matter. If selection is acting on epistatic interactions rather than additive gene effects, the breeder's equation will give you misleading predictions. I ran into this exact problem when working with a crop improvement program. We had strong selection differentials for yield but the response was consistently lower than predicted. The culprit turned out to be a significant epistatic component we hadn't accounted for. Once we switched to a genomic selection model that included interaction terms, our predictions aligned much better with observed outcomes. The total process time for model refinement was about three weeks, and it saved us from making planting decisions based on faulty expectations.

When selective pressures fail to produce evolution
Selection requires variation. If a population is genetically uniform, no amount of selective pressure will produce evolutionary change. This is why endangered species with low genetic diversity are vulnerable even when the selective pressures they face haven't changed. They lack the raw material for adaptation. Gene flow can overwhelm local selection. If migrants arrive frequently from a population adapted to different conditions, their genes dilute local adaptation. This is a common problem in conservation when fragmented populations need to be connected but the source population isn't well matched to the local environment. The resulting hybrid swarms can be maladapted to both source and recipient conditions. Genetic drift can dominate in small populations. When population size is small, random changes in allele frequency can override selection. A beneficial allele can be lost by chance, and a deleterious one can fix. This is particularly relevant for populations going through bottlenecks, which many species do when habitat is destroyed or fragmented. The bottleneck effect reduces variation and increases the role of drift, making recovery slower than you would expect from selection alone.
There is also the issue of maladaptation to novel pressures. Humans have created selective pressures that many organisms haven't encountered before in their evolutionary history. Pesticides, antibiotics, heavy metals, and synthetic chemicals act as intense selective pressures on timescales much shorter than most species can adapt to. This is why antibiotic resistance evolves so quickly in bacteria. The generation time is short, the mutation rate is high, and the selective pressure is direct and unavoidable. The result is a public health crisis that no amount of traditional conservation strategy can address.
A note on prediction and uncertainty
Predicting evolutionary responses is possible but it comes with significant uncertainty. The main sources of error are inaccurate heritability estimates, unmeasured correlated traits, changing environments, and gene-environment interactions. Even with good data, predictions are probabilistic, not deterministic. Two identical populations under identical selective pressures can evolve differently due to stochastic events, especially if they are small. For practical applications like agriculture, medicine, and conservation, the best approach is to combine theoretical modeling with empirical monitoring. Models give you a framework and initial predictions. Empirical data tells you whether you are wrong and how wrong. Iterating between the two is the only reliable method. I have seen projects waste years by committing to a single model without updating it as new data came in. That is not how evolution works, and it shouldn't be how you study it either. The bottom line is that selective pressures are everywhere and they are always acting. The ones you can see are the loud ones. The quiet ones, the ones that barely shift allele frequencies by a fraction of a percent each generation, are the ones that matter most over the long term. You don't need to force them to do their work. They already know what to do.