Cellular Respiration Products: The Actual Breakdown
When you strip away the simplified diagrams in introductory biology textbooks, cellular respiration yields three primary products: carbon dioxide, water, and adenosine triphosphate (ATP). That's it. Everything else is just intermediate states or byproducts that get recycled mid-process. The overall chemical equation is straightforward—C6H12O6 + 6O2 6CO2 + 6H2O + ATP—but running that reaction inside an actual cell is where the complications start. Most people stop at ATP as "the product" and move on, which is technically correct but missing half the picture. Let me walk through what actually comes out of each stage and why the numbers on paper rarely match reality.
What Are The Products Of Cellular Respiration
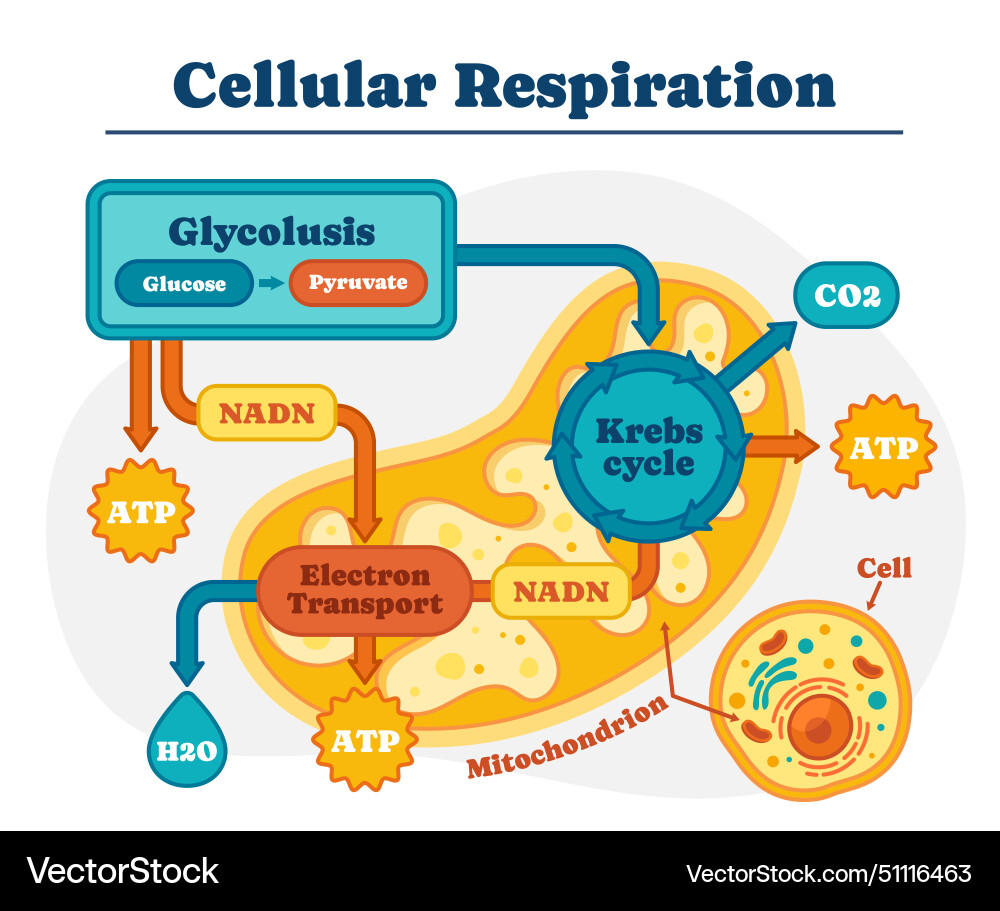
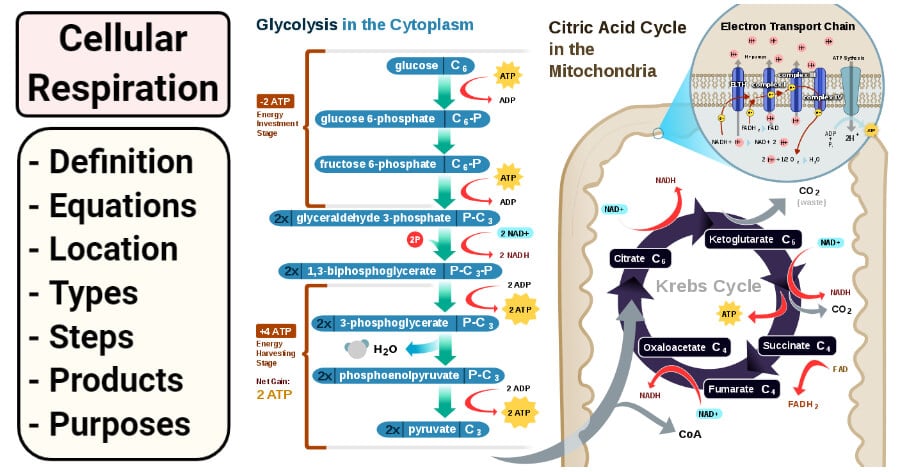
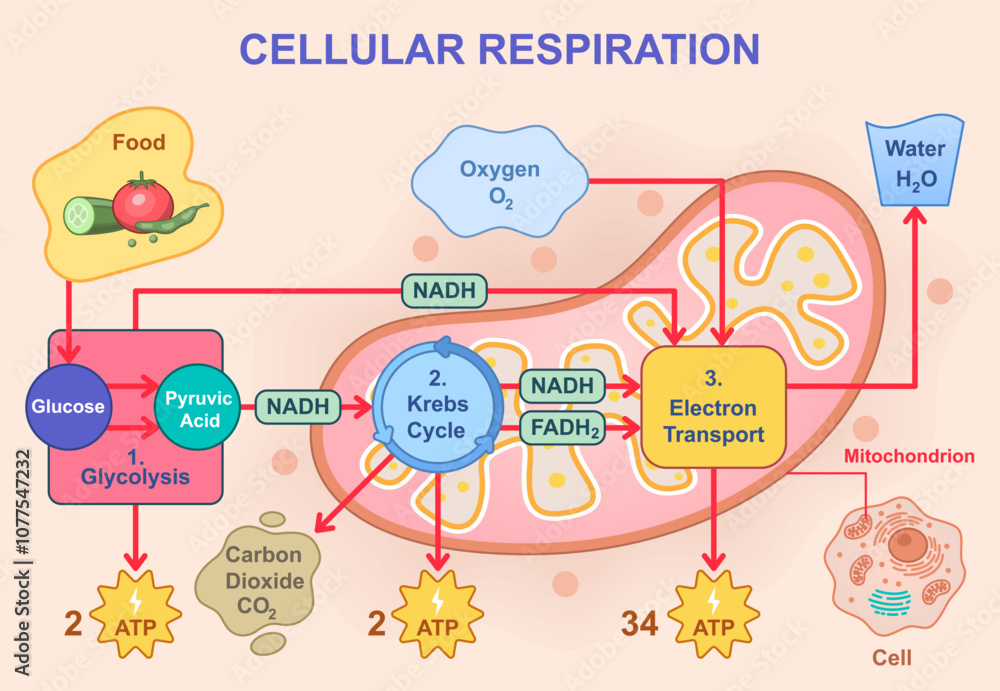
Breaking it down by stage. Glycolysis happens in the cytoplasm and produces 2 net ATP, 2 NADH, and 2 pyruvate molecules from one glucose. No oxygen required here, which is why cells can still partially function when things go south. The pyruvate then feeds into the pyruvate dehydrogenase complex, converting each one into acetyl-CoA while releasing one CO2 per pyruvate—that's two CO2 molecules total so far, and the NAD+ gets reduced to NADH in the process. The citric acid cycle, also called the Krebs cycle or TCA cycle, runs in the mitochondrial matrix. Each acetyl-CoA produces 3 NADH, 1 FADH2, 1 GTP (which converts to ATP), and 2 CO2. Since you start with two acetyl-CoA from one glucose, that's double those numbers. By the time you finish this stage, you've made another 2 ATP equivalent and released 4 more CO2 molecules. So add it up: 6 CO2 total from the full oxidation of one glucose, 2 from glycolysis via the link reaction, and 4 from the citric acid cycle. The water comes from the electron transport chain, not from any of these earlier stages. The electron transport chain and oxidative phosphorylation are where the bulk of ATP gets generated. NADH and FADH2 dump their electrons into complexes I through IV, pumping protons across the inner mitochondrial membrane. The proton gradient drives ATP synthase, which produces roughly 26 to 28 additional ATP per glucose. Oxygen sits at the end of the chain as the final electron acceptor, combining with electrons and protons to form water. That's where the H2O product comes from. Total ATP yield per glucose molecule under ideal conditions is approximately 30 to 32, though this number varies depending on the shuttle system your cell uses to get cytoplasmic NADH into the mitochondria.
I spent months troubleshooting yeast fermentation assays in grad school, and one thing that always caught students off guard was the gap between theoretical and actual ATP yield. The textbook says 36 or 38 ATP depending on which edition you're using, but real measurements in living systems consistently come in lower. The reason isn't that the math is wrong—it's that the proton gradient leaks. Protons cross the inner mitochondrial membrane without going through ATP synthase, a phenomenon called proton leak or uncoupling. This is actually a feature, not a bug. Brown fat uses controlled uncoupling to generate heat instead of ATP. In most other cell types, proton leak accounts for maybe 20 to 30 percent of the gradient, which explains why your real-world yield sits around 30 to 32 instead of the theoretical maximum. Another thing nobody emphasizes enough: the NADH from glycolysis sits in the cytoplasm, and it can't cross the inner mitochondrial membrane directly. Your cell has to use shuttle systems. The malate-aspartate shuttle transfers those electrons efficiently and yields about 2.5 ATP per NADH. The glycerol-3-phosphate shuttle is less efficient and effectively converts that NADH to FADH2, yielding only about 1.5 ATP per original NADH. Different tissues use different shuttles. Liver and heart prefer the malate-aspartate route. Skeletal muscle and brain lean toward the glycerol-3-phosphate shuttle. If you're calculating yield for a specific tissue, picking the wrong shuttle throws off your entire accounting. There are also non-ATP products worth tracking. Reactive oxygen species, particularly superoxide and hydrogen peroxide, are generated as inevitable byproducts when electrons leak from complexes I and III during normal respiration. Most get neutralized by superoxide dismutase and catalase, but under stress or with certain toxins, this cleanup system gets overwhelmed. That's not a product the cell wants, but it's a direct consequence of the chemistry involved.
Get the Full Details

If you're working with isolated mitochondria and measuring respiration rates, you'll notice that adding an uncoupler like FCCP collapses the proton gradient and maxes out electron flow. Oxygen consumption spikes, ATP production drops to near zero, and heat becomes the primary output. This is actually how some pesticides and dietary supplements exert toxic effects—they artificially uncouple the system. Understanding this helps explain why simply counting ATP molecules doesn't tell the whole story of what the process produces under different conditions. For practical purposes in a lab setting, if you need to quantify respiration products, CO2 evolution and O2 consumption are the easiest to measure directly. You can use a Clark-type oxygen electrode for dissolved O2 and an infrared CO2 analyzer for gas exchange. From the respiratory quotient—the ratio of CO2 produced to O2 consumed—you can infer what substrate the cell is burning. A ratio of 1.0 means pure carbohydrate oxidation. Around 0.7 indicates fat metabolism. Values between 0.8 and 0.85 suggest mixed fuel sources or protein involvement. This is useful when you're trying to figure out what's happening metabolically without running a full spectrometry panel. One edge case that cost me about three weeks of confused data early on: when cells switch to anaerobic metabolism, the products change entirely. Instead of CO2 and water and lots of ATP, you get lactate (in animal cells) or ethanol and CO2 (in yeast), plus only that baseline 2 ATP from glycolysis. The electron transport chain stops because there's no oxygen to accept electrons, NADH backs up, and the cell has to regenerate NAD+ through fermentation to keep glycolysis running at all. It's not a failure state for single-celled organisms or for muscle cells during brief intense effort. It's a backup system. But if you're measuring cellular respiration products and your sample has been hypoxic, you'll see lactate accumulating and your ATP yield will be a fraction of what the aerobic numbers suggest. Always check your oxygen levels before drawing conclusions from respiration data.