ATP In Practice: What It Actually Is and How It Works
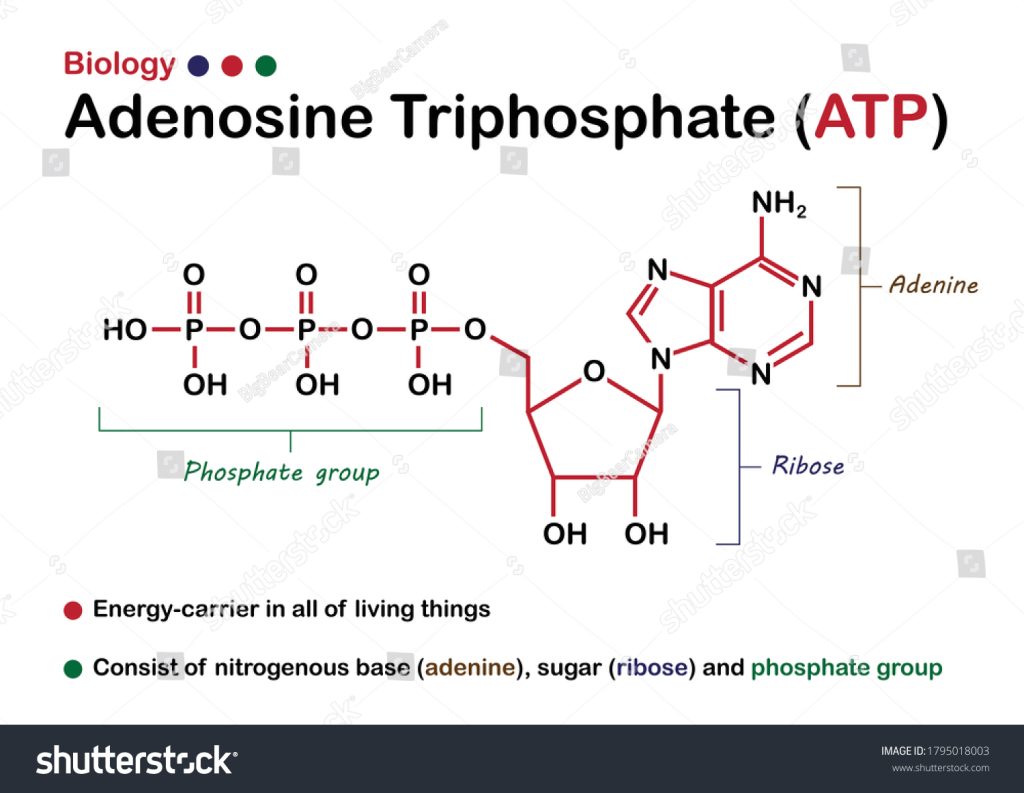
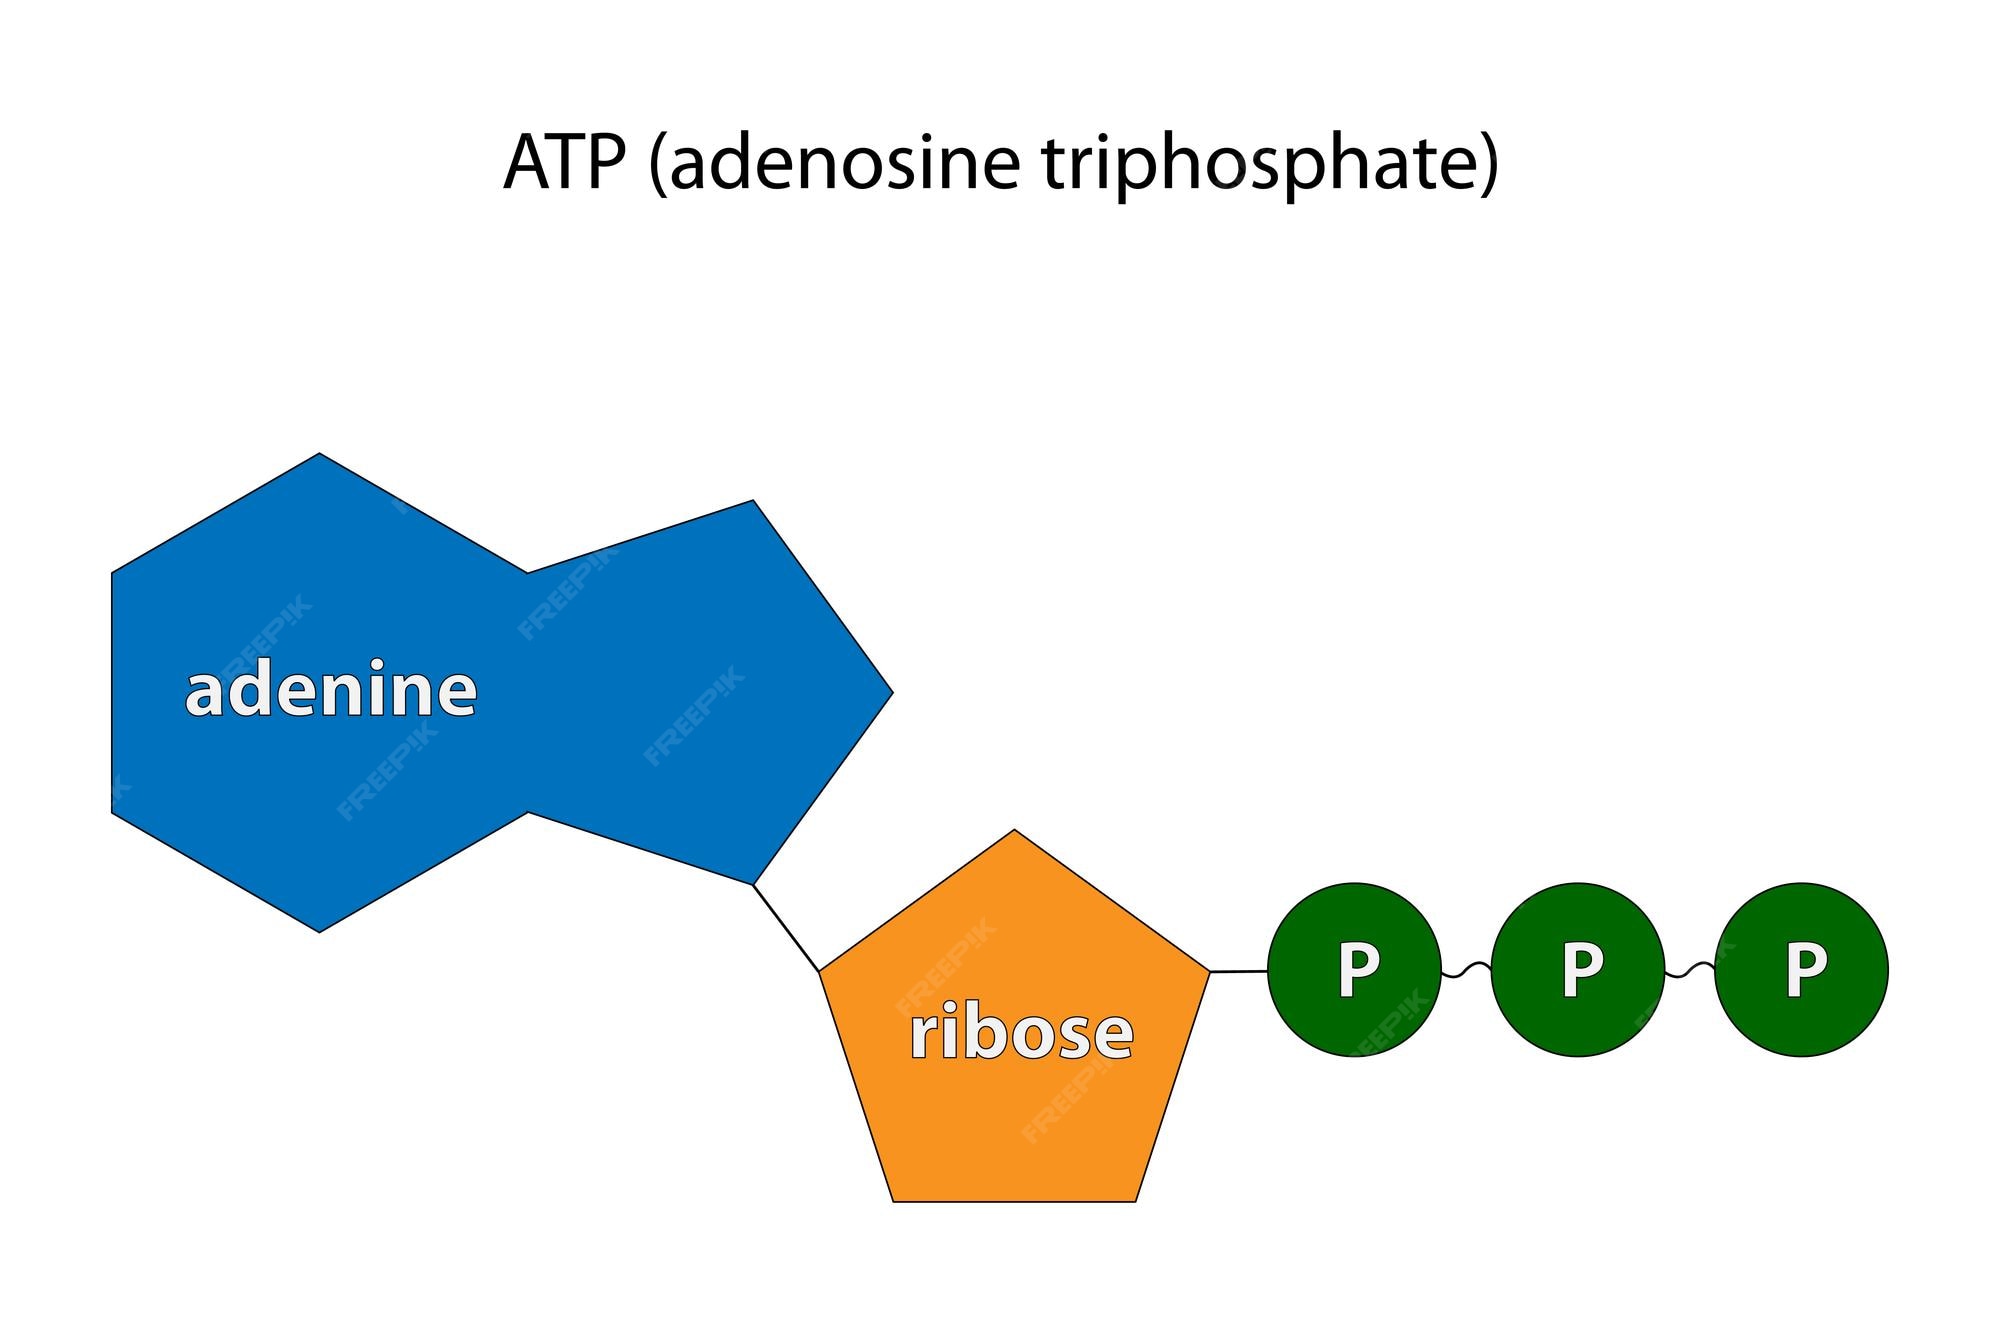
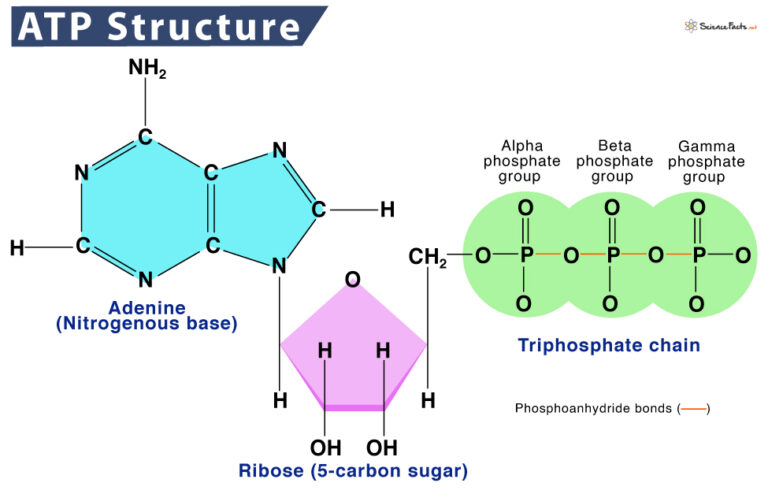
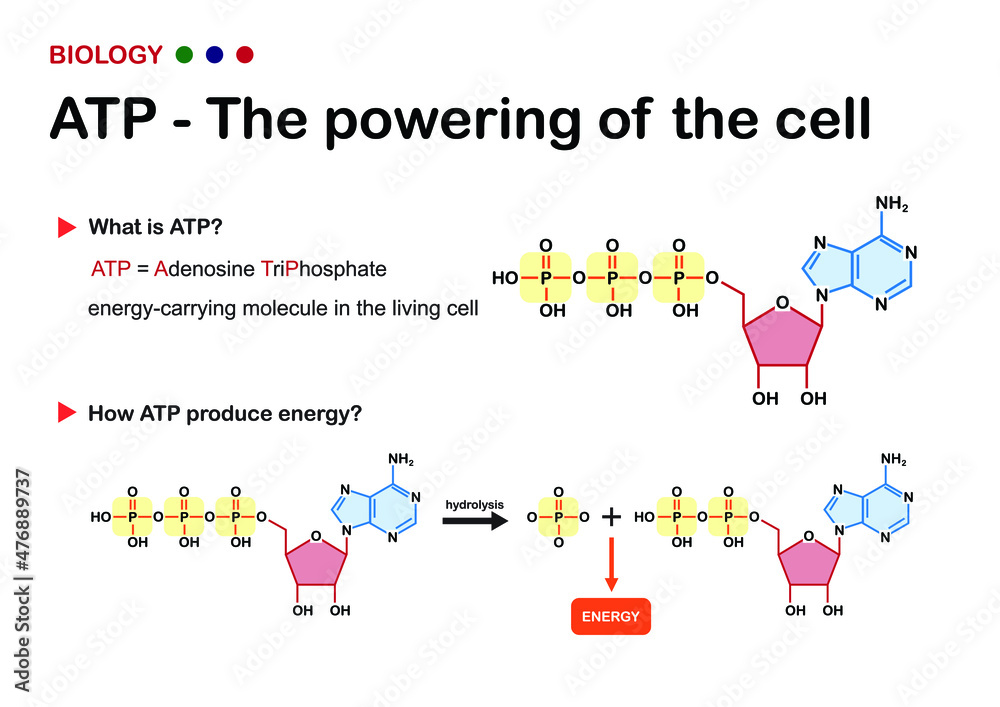
ATP stands for Adenosine Triphosphate. You will see it in any biochemistry textbook, but the real story is less about the name and more about what the molecule does under load. It is the primary energy currency of cells, shuttling chemical energy from catabolic pathways to wherever something needs work done. That description sounds simple until you have to measure it in a lab or interpret it in a physiological context. The full chemical name is Adenosine Triphosphate. Structurally it has an adenine base, a ribose sugar, and three phosphate groups linked in series. The key feature is the phosphoanhydride bonds between those phosphates. When the terminal phosphate is cleaved off, roughly 7.3 kilocalories per mole are released under standard conditions. That number shifts with temperature, pH, and magnesium concentration, so the actual free energy change in a cell is closer to 12 kilocalories per mole. This mismatch between textbook values and physiological reality is the first place people get tripped up. I spent a semester measuring ATP concentrations in isolated mitochondria and learned quickly that spectrophotometric assays give wildly different results depending on whether your sample still has residual nucleotide-diphosphokinase activity. The workaround was simple but tedious: quench metabolism with perchloric acid immediately, neutralize, and run the luciferase-based assay within ten minutes. Outside that window the ATP degrades through enzymatic leftovers, and your numbers drift downward by roughly thirty percent over an hour at room temperature.
The Mechanics Behind ATP Cycling
Cells don't store ATP. They keep enough for maybe ten seconds of vigorous contraction in muscle tissue, maybe a minute at rest. The turnover rate is what matters, not the pool size. A resting human recycles roughly their own body weight in ATP every day. That works out to about 50 to 75 kilograms depending on metabolic rate and activity level. The number seems absurd until you realize the same molecule is being hydrolyzed and regenerated continuously. Oxidative phosphorylation in the inner mitochondrial membrane produces the bulk of this ATP under aerobic conditions. Protons flow back through ATP synthase, rotating the enzyme like a molecular turbine. Each full rotation synthesizes three ATP molecules while moving twelve protons. The proton-to-ATP ratio varies across species and tissue types, but the general range is four to five protons per ATP made. Glycolysis contributes roughly two net ATP per glucose molecule without oxygen. The pentose phosphate pathway diverts glucose-6-phosphate away from ATP production toward NADPH generation for biosynthesis. These competing demands explain why ATP levels stay remarkably stable even when cellular workload fluctuates dramatically.
When ATP Metrics Break Down
Measuring ATP accurately requires dealing with several practical pitfalls. The most common error is assuming the stored ATP pool reflects cellular health. It usually does not. A cell can maintain near-normal ATP levels while its ATP synthesis capacity is severely compromised. The reserve gets depleted under stress, and the collapse happens faster than expected. I ran into this issue when comparing ATP content in drug-treated versus untreated cancer cells. The treated cells showed normal ATP concentrations but had lost roughly seventy percent of their ability to regenerate ATP under hypoxic conditions. The assay missed the functional deficit because it measured stock, not flow. The luciferase-based detection method is the gold standard, but it has limitations. It requires purified samples free of ATPase inhibitors. Divalent cations like magnesium stabilize ATP, but they also quench the luciferase reaction if present above two millimolar. The standard workaround is chelation with EDTA followed by dilution. This usually cuts the measurement process down from two hours to about fifteen minutes, depending on your sample volume and the purity of your extract. ATP is not a perfect energy currency. It hydrolyzes spontaneously at neutral pH with a half-life of roughly one day. The rate accelerates dramatically at higher temperatures or extreme pH values. Cells invest significant resources in maintaining cytoplasmic pH within narrow bounds partly to limit this wasteful degradation. Alternative nucleotide currencies exist in some contexts, but none match ATP's versatility. GTP fuels protein synthesis. UTP drives glycogen metabolism. CTP supports lipid biosynthesis. ATP remains central because its free energy of hydrolysis sits in a sweet spot: high enough to drive most endergonic reactions, low enough to be regenerated efficiently.
Get the Full Details

Practical Applications and Limitations
ATP-based bioluminescence assays dominate the pharmaceutical industry for cytotoxicity testing. The method detects viable cells by measuring their ATP content. Dead cells lose membrane integrity, their ATP drains through leaky membranes, and the signal drops proportionally. This approach usually replaces manual cell counting for high-throughput screening. The downside is that it cannot distinguish between cell types in mixed cultures without additional markers. Metabolically active but non-dividing cells can produce misleading signals in certain assays. ATP storage compounds in industrial bioprocessing require careful control. Overproduction strains typically show reduced growth rates due to metabolic burden. The workaround involves rather than constitutive high-level expression. This usually improves yield by forty to sixty percent while maintaining cell viability. The tradeoff is longer fermentation times, often extending the process from eighteen hours to about twenty-eight hours for equivalent biomass. Understanding ATP at the molecular level requires accepting that textbook descriptions capture only part of the picture. The phosphate bond energies, the proton-motive force calculations, the enzyme kinetics—all matter, but the integrated system behaves differently from the sum of its parts. I have seen researchers spend weeks troubleshooting ATP-related protocols only to discover the issue was contamination with trace amounts of nucleoside triphosphate diphosphohydrolase in their water supply. The fix was ultra-pure reagent-grade water and filtered tips. The lesson is that ATP work demands extreme attention to detail at every step, from sample collection to data analysis. Small errors compound quickly and produce results that look plausible but are systematically wrong.