Evolution Isn't What Most People Think It Is
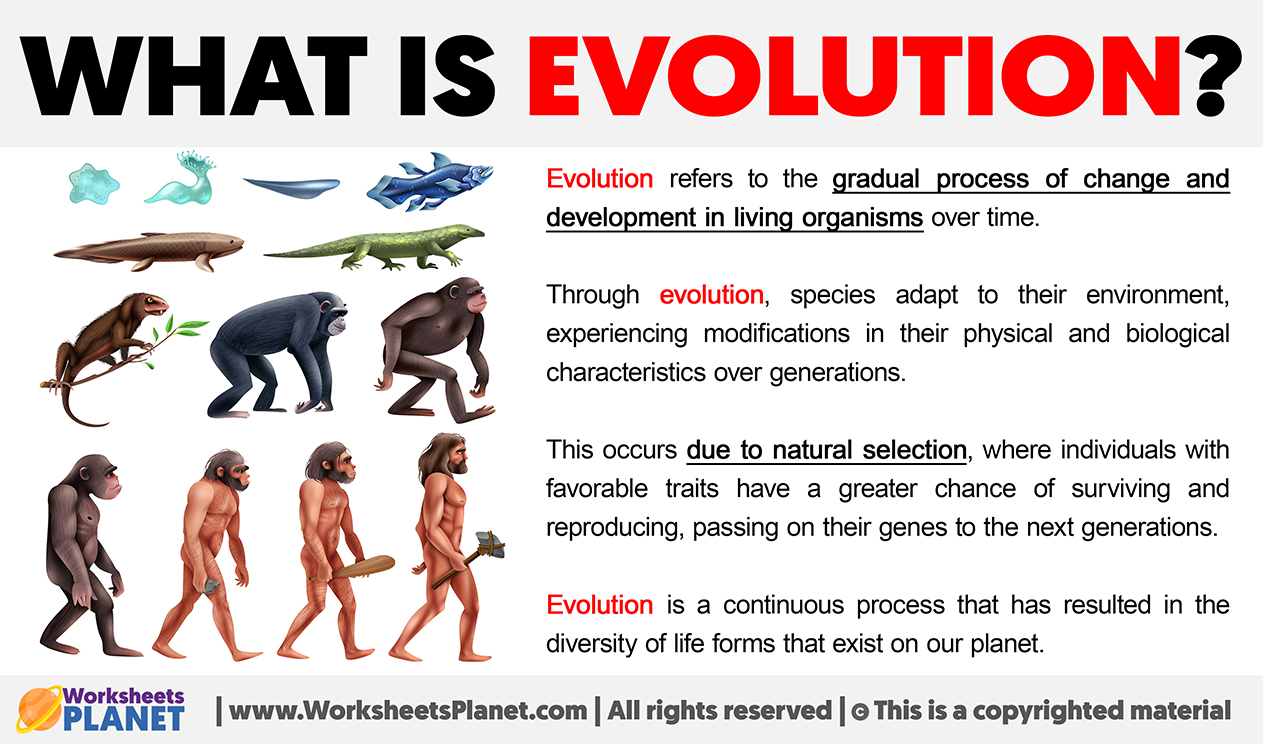
Evolution is simply the change in allele frequencies within a population over successive generations. That's it. A technical definition, but a complete one. The popular understanding has morphed into something wilder than the actual mechanism — a narrative of progress, of organisms striving toward improvement. Neither striving nor improvement are required components. You can watch evolution operate in a petri dish with bacteria exposed to antibiotics. You can also watch it fail to produce anything resembling complexity when the selection pressure doesn't favor it. The four mechanisms are mutation, genetic drift, gene flow, and natural selection. They interact constantly. Mutation introduces new variants. Genetic drift shifts frequencies randomly, especially in small populations. Gene flow moves alleles between populations through migration. Natural selection amplifies or reduces alleles based on differential reproductive success. Most introductory textbooks present these as separate boxes. In practice they overlap and compete, sometimes within the same generation.
What Does Evolution Mean When the Math Doesn't Lie
I spent years working with microbial evolution experiments, specifically tracking how Pseudomonas fluorescens adapts under constant environmental stress. The setup is straightforward: serial passage into fresh medium, measure fitness changes over hundreds of generations. The results are never clean. One strain I was monitoring developed a mutation in the rpoB gene that conferred resistance to a particular phage, but it carried a steep metabolic cost. In the presence of the phage, the mutant dominated within forty-eight hours. Remove the phage, and the wild-type outcompeted it within six hours. The allele frequency curve didn't show a clean trajectory. It oscillated. This is the part people miss when they're looking for a linear story. Evolution doesn't optimize. It navigates a fitness landscape where peaks shift because the landscape itself changes. A mutation that looks beneficial today might become neutral or deleterious tomorrow if the environment shifts. The classic example is sickle cell trait and malaria resistance — heterozygote advantage that maintains both alleles in the population. Remove the malaria pressure, and the balance tips. The alleles don't disappear from the gene pool immediately because drift and gene flow keep reintroducing them, but the selection pressure that maintained them is gone. Another counter-intuitive point: most evolutionary change happens through standing genetic variation rather than new mutations. When a population faces a novel stressor, the alleles that confer resistance often already exist at low frequency. A new beneficial mutation is theoretically possible, but the probability of it arising and fixing before the population goes extinct is slim in most realistic scenarios. This means conservation biologists should prioritize maintaining large effective population sizes — not because diversity sounds good in a mission statement, but because standing variation is the actual raw material that selection works with when things go wrong.
The bottleneck effect demonstrates this bluntly. A population crashes to a small number of individuals, and the surviving gene pool is a random subset of the original. Alleles that were common before can vanish entirely. Rare alleles might become common purely by chance. The cheetah is the textbook case — extremely low genetic diversity resulting from a historical bottleneck, which makes the species vulnerable to disease outbreaks and reduces reproductive success. But here's the nuance: low diversity doesn't mean the population is doomed. It means the population has limited capacity to respond to novel selective pressures. If the environment stays relatively stable, a depauperate gene pool is functional. It's a loaded question mark when conditions change. Gene flow is another mechanism that gets misunderstood. People assume more mixing is always better for genetic health. It usually is, but not universally. Local adaptation can be swamped by excessive gene flow from populations adapted to different conditions. I've seen this in fragmented habitats where corridors connecting isolated populations resulted in maladapted hybrids because the source population carried alleles suited to a completely different microclimate. The connectivity improved short-term diversity metrics but eroded local adaptation over several generations. The workaround in those situations is directional breeding programs or assisted migration rather than simple corridor construction. Molecular evolution and phenotypic evolution don't always move in sync. Neutral theory predicts that most molecular changes are fixed by drift rather than selection. The Kimura neutral model estimates that roughly 90 percent of nucleotide substitutions in non-coding regions are selectively neutral. This means you can observe substantial genetic divergence between populations or species without any observable phenotypic change. The molecular clock is useful for dating splits but unreliable for inferring functional change. Two populations might show 5 percent sequence divergence in a particular gene while looking identical in morphology and behavior.
Get the Full Details

Epistasis complicates predictions even further. The effect of a mutation depends on the genetic background in which it appears. A variant that's beneficial in one genotype might be neutral or harmful in another. This non-additive interaction means evolutionary trajectories are path-dependent. The order in which mutations accumulate matters. Crossing a fitness valley — a sequence of genotypes where intermediate steps are less fit than the starting and ending points — is theoretically possible through drift in small populations but statistically unlikely in large ones. I ran simulations where populations of 10,000 never crossed a particular valley, but populations of 500 did, purely because drift allowed them to sample genotypes that selection would have purged in the larger group. Here's the practical implication for anyone working with evolutionary concepts: the timescale changes everything. Microevolution — allele frequency shifts within a population — is observable in real time. Industrial melanism in peppered moths, pesticide resistance in insects, antibiotic resistance in bacteria. Macroevolution — speciation and major morphological transitions — operates on geological timescales and leaves an incomplete record. The fossil record is biased toward hard-bodied organisms in aquatic environments. Soft-bodied organisms and terrestrial species are vastly underrepresented. This gap doesn't invalidate evolutionary theory. It means certain claims about specific transitional forms are harder to verify empirically, and legitimate uncertainty exists about the exact sequences of morphological change in lineages with poor fossil representation. Convergent evolution is another area where intuition fails. Similar environmental pressures produce similar adaptations in unrelated lineages — sharks and dolphins both evolved streamlined bodies and dorsal fins, but their last common ancestor didn't have either structure. This happens because physics and chemistry constrain the space of possible solutions. It doesn't mean evolution has a goal. It means certain functional problems have limited viable answers, and different lineages independently discover the same answers through different genetic pathways.
If you're trying to apply evolutionary thinking to a practical problem — whether that's managing a threatened species, designing an antibiotic rotation protocol, or understanding pathogen emergence — the first step is identifying the relevant population size, the selection pressure, and the timescale. Those three variables determine whether drift or selection dominates, whether standing variation or new mutation matters more, and whether you're likely to observe change within a human-relevant timeframe. Everything else builds from there.