The Light Reactions First
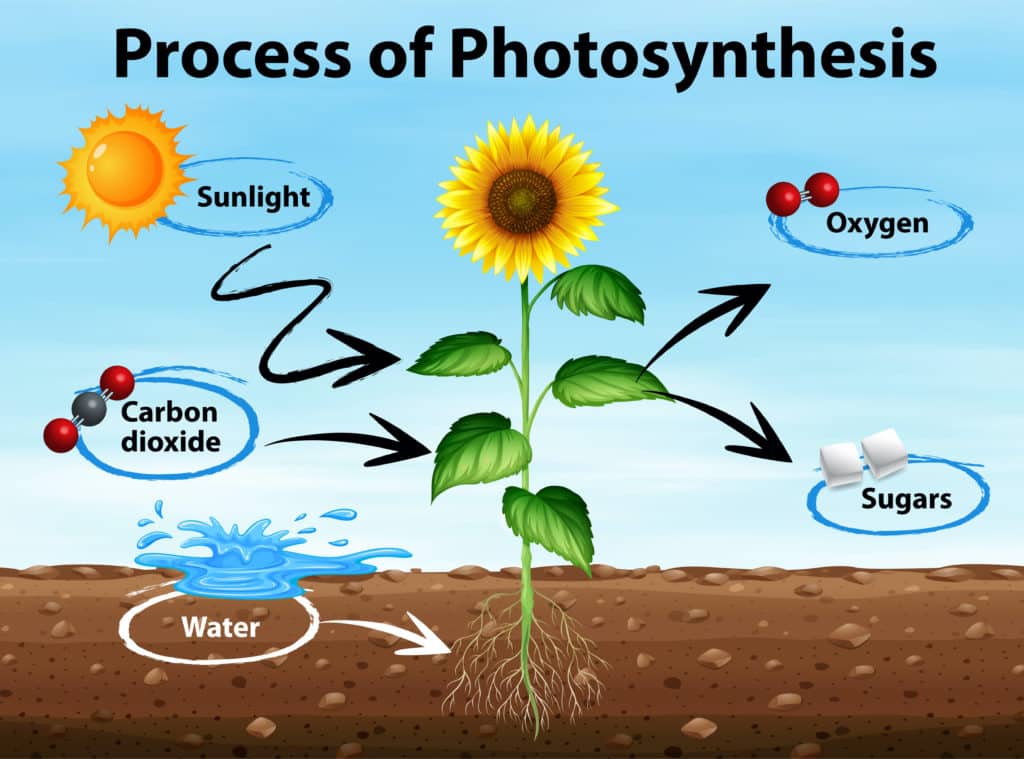
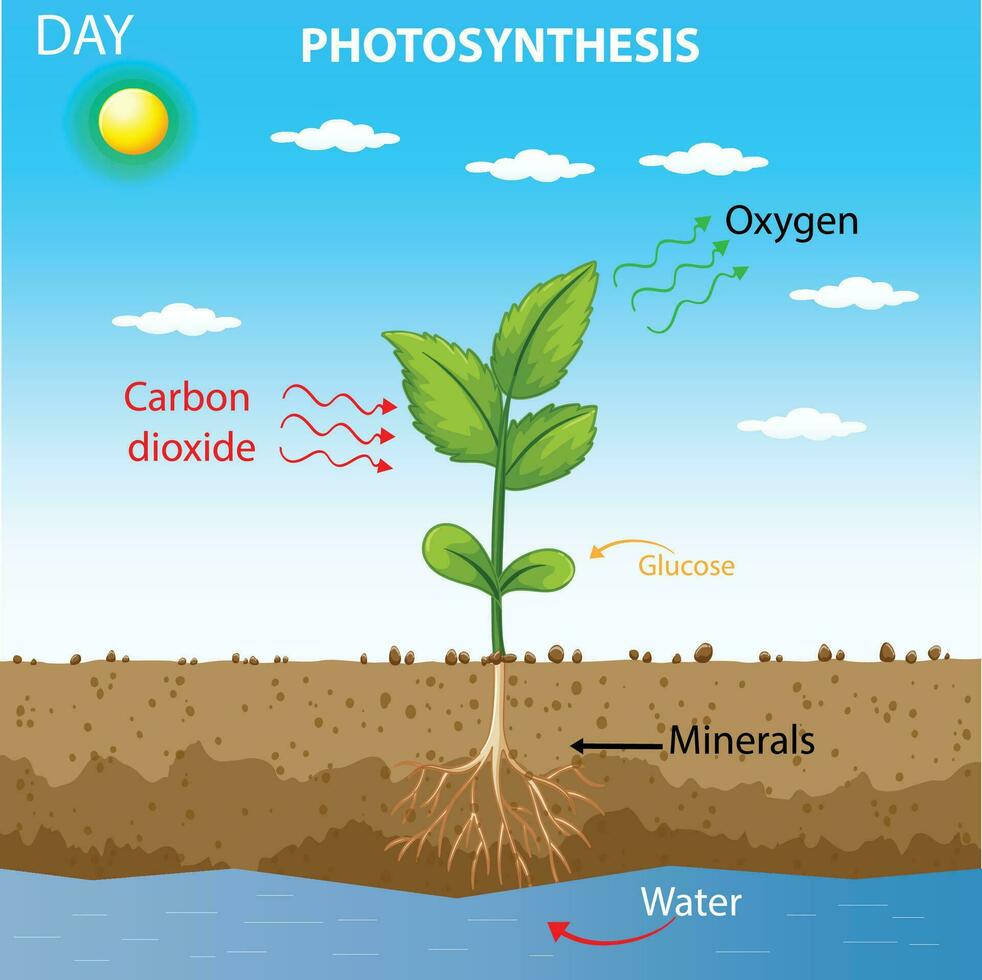
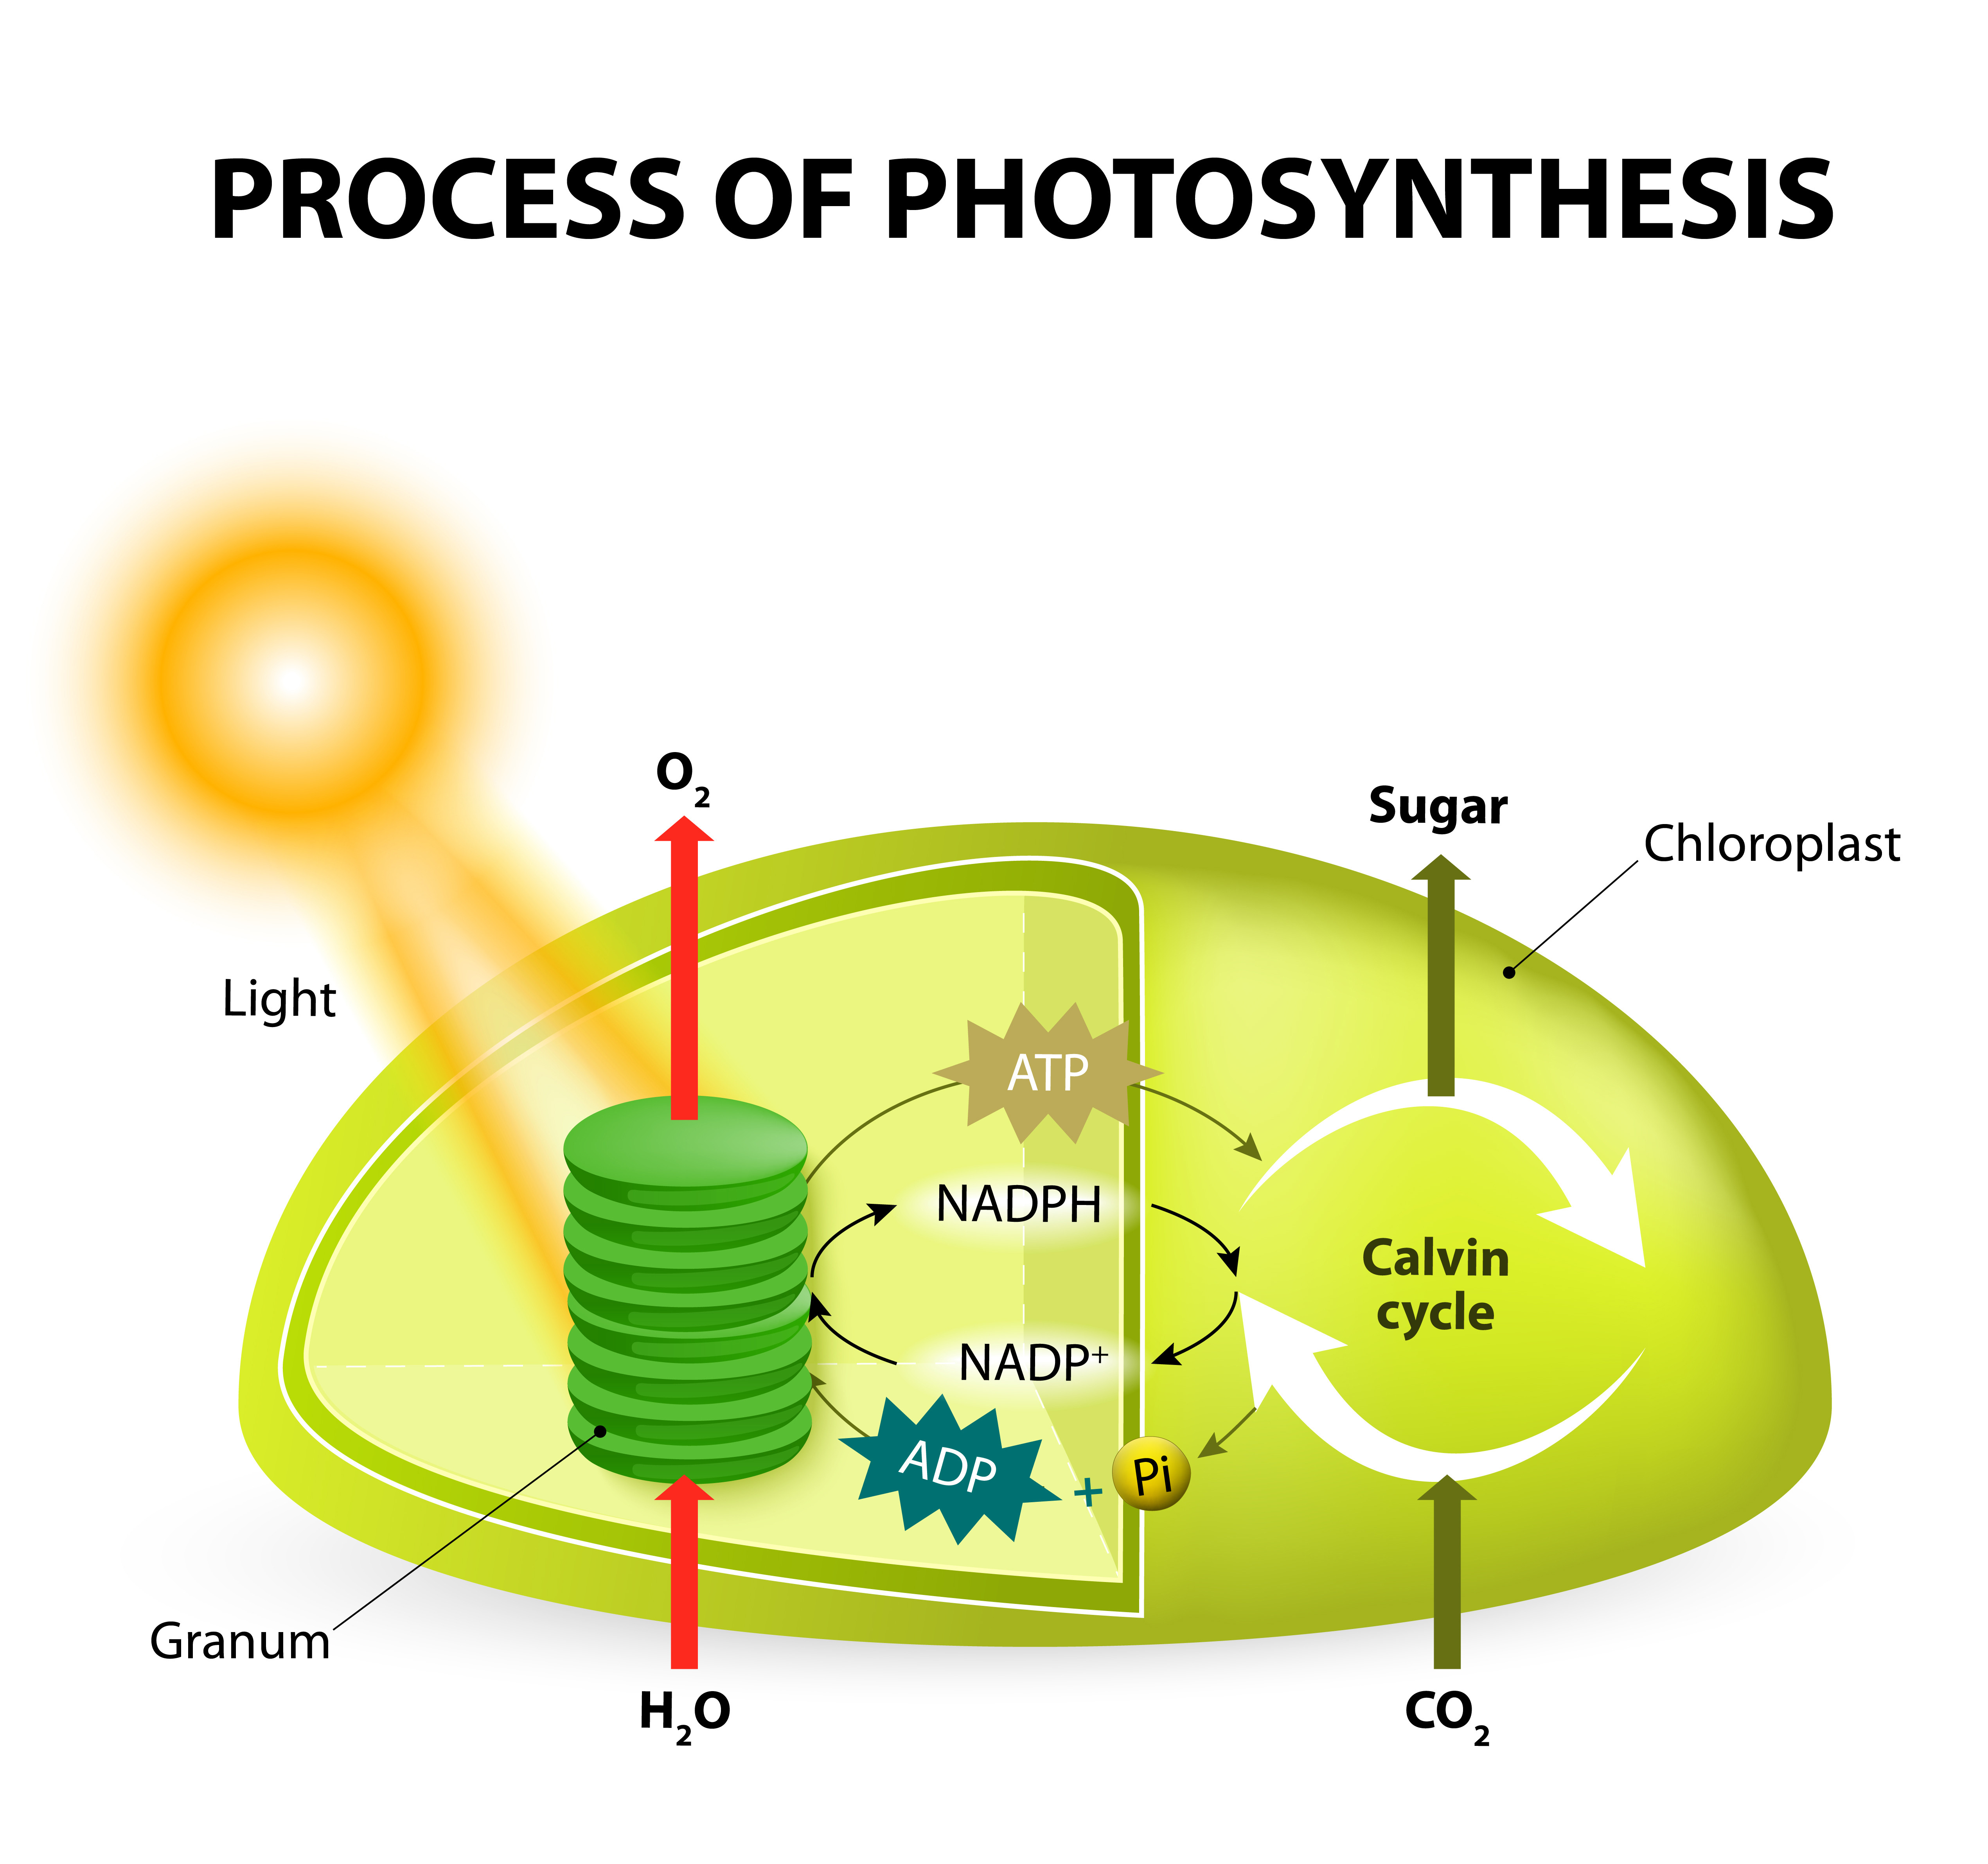
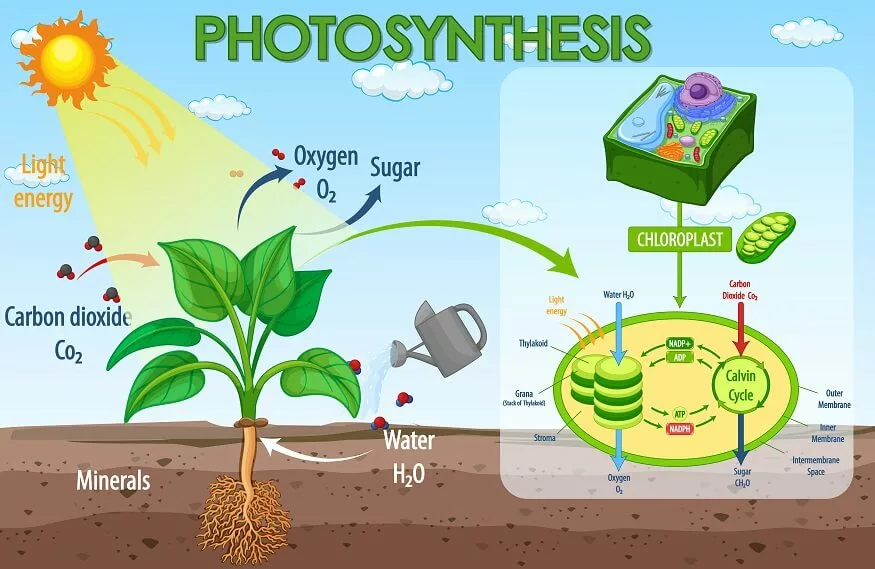
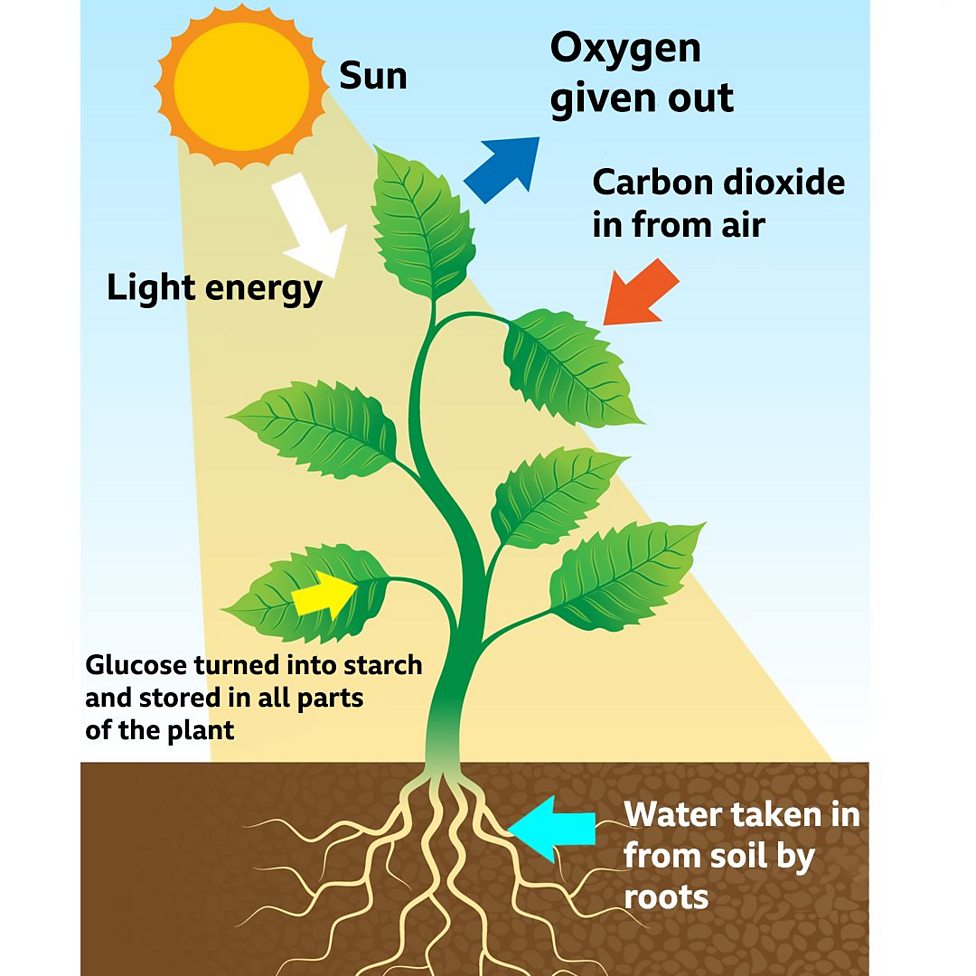
Photosynthesis splits water molecules using photon energy captured by chlorophyll in the thylakoid membranes. The immediate output is a proton gradient across that membrane, which drives ATP synthase to produce ATP, while the electrons reduce NADP+ to NADPH. Both molecules carry chemical energy but serve different roles — ATP powers short-term cellular work, and NADPH acts as a high-energy electron carrier feeding the next phase. Oxygen is released as a byproduct when water is split. It's not the goal of the process. Plants don't produce oxygen to help animals. It's just what's left over. I once calibrated a gas exchange system on a greenhouse-grown batch of sugar beets and kept getting inconsistent O2 evolution rates. Turned out the leaves were partially senescent near the base, and older tissue has a much higher mitochondrial respiration rate that consumes some of the oxygen right as it's produced. The net output dropped significantly compared to what the models predicted. I had to isolate young, fully expanded leaves and account for a dark respiration baseline before trusting the gross photosynthetic rate numbers.
What Does Photosynthesis Make
The direct carbon product of the Calvin cycle is glyceraldehyde-3-phosphate, commonly called G3P. This is a three-carbon sugar phosphate. Two molecules of G3P exit the cycle and can be combined to form one molecule of glucose-6-phosphate. From there the plant can synthesize sucrose for transport through the phloem, starch for storage in chloroplasts or specialized organs, or cellulose for cell wall construction. What ends up in the fruit versus the root versus the wood depends entirely on the plant's developmental stage and environmental conditions. A common mistake people make is thinking photosynthesis makes glucose as the main end product. Glucose is an intermediate. It's rarely accumulated in free form because it's osmotically active and would draw too much water into the chloroplast. The plant immediately converts it to sucrose or starch. If you're measuring carbohydrate accumulation in a lab setting, you need to decide which form you're quantifying and use the appropriate assay. Anthrone for total carbohydrates, phenol-sulfuric acid for sugars, and iodine staining for starch. Each gives you different information.
The Calvin-Benson Cycle in Practice
Rubisco fixes atmospheric CO2 onto ribulose-1,5-bisphosphate, a five-carbon acceptor molecule. The resulting six-carbon intermediate immediately splits into two molecules of 3-phosphoglycerate. These get phosphorylated by ATP and reduced by NADPH to form G3P. Most of the G3P recycles back through a series of reactions that regenerate RuBP, but a fraction leaves the cycle to build carbohydrates. The cycle turns twelve times to produce one net G3P that exits. The thing nobody emphasizes enough is how much energy this actually costs. Fixing one molecule of CO2 requires three ATP and two NADPH. That means producing one G3P molecule costs eighteen ATP and twelve NADPH. For a C3 plant growing under typical conditions, light saturation occurs around 1000 to 1500 micromoles of photons per square meter per second. Beyond that, the extra light energy can't be used productively and starts causing photoinhibition, damaging the D1 protein in photosystem II. I've seen growers run LED arrays at full intensity in indoor setups and wonder why growth plateaued and leaf margins started chlorosing. The problem wasn't insufficient light. It was too much.
Get the Full Details
C4 and CAM Aren't Just Textbook Footnotes
C4 plants like maize and sorghum spatially separate the initial CO2 fixation from the Calvin cycle. They fix CO2 into oxaloacetate using PEP carboxylase in mesophyll cells, then shuttle that carbon as malate into bundle sheath cells where Rubisco operates in a CO2-enriched environment. This dramatically reduces photorespiration, which becomes a serious problem for C3 plants at high temperatures and low CO2 concentrations. Photorespiration can consume up to twenty-five percent of the fixed carbon in a C3 plant on a hot, dry day. That's carbon going nowhere, producing no sugar, just burning through energy. CAM plants like agave and pineapple take temporal separation instead. They open their stomata at night to fix CO2 into malate, storing it in vacuoles, then run the Calvin cycle during the day with stomata closed. The tradeoff is enormous. CAM photosynthesis typically fixes only about one-fifth the carbon per unit time compared to C3 plants under comparable conditions. But in arid environments where water loss through transpiration is the limiting factor, that's an acceptable compromise. I worked with a research team growing Sedum for phytoremediation trials and had to calibrate their gas exchange measurements differently because standard C3 models completely overestimated their daytime carbon uptake. The nocturnal CO2 fixation meant we needed overnight sampling to get accurate assimilation rates.
What Actually Determines the Output
Light intensity, CO2 concentration, temperature, and water availability are the four main drivers, but they interact in ways that aren't straightforward. Increase CO2 from ambient levels and C3 plant rates can jump substantially until another factor becomes limiting. Raise the temperature and enzymatic rates speed up initially, but Rubisco's affinity for CO2 drops while its oxygenase activity increases, making photorespiration worse. At extreme temperatures the thylakoid membrane structure begins to break down and electron transport stalls. Water stress closes stomata to prevent desiccation, which cuts off CO2 supply even if light and temperature are ideal. Under these conditions the plant shifts into maintenance mode, prioritizing protein repair and osmoprotectant synthesis over growth. The carbohydrate output drops sharply. If you're trying to predict biomass accumulation from photosynthetic parameters, you need to know which factor is currently limiting. Liebig's law of the minimum still applies here — growth is controlled by the scarcest resource, not the total available resources.